Invasive species’ spread facilitated by inconsistent approaches

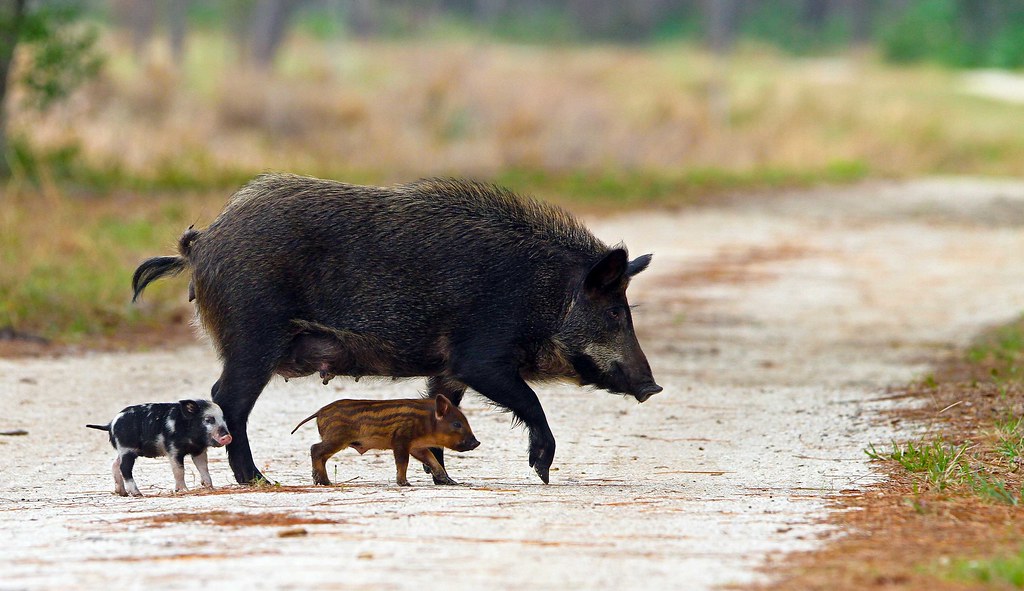
feral hogs — one the invasive species on which state approaches vary; photo by Creg Oneal via Flickr

Several groups of scientists are addressing systemic problems that impede efforts to counter bioinvasions. One of those problems is the lack of a consistent approach in federal systems. 

Drake et al. (2026) (full citation at the end of this blog) evaluate the impacts of this situation in the United States where – they argue – the national government has been slow to adopt overarching policies and provide adequate and dependable funds to implement them. The result is a patchwork of varying – even clashing – regulations and differing levels of effort that undermine program efficacy. Conflicting approaches add to such well-known challenges as limited budgets and evolving goals. They recommend applying such existing frameworks as the National Invasive Species Council’s (NISC) Early Detection / Rapid Response framework or One Biosecurity to facilitate integration and cooperation among the large variety of sectors affected. (NISC’s purpose is to coordinate federal agencies’ programs. The Council has no official role vis a vis state programs. Still, there is no legal impediment to states adopting any NISC approach which they consider appropriate.) At the same time Drake et al. (2026) warn against imposing too great uniformity or lacking flexibility.

I regret that Drake et al. (2026) do not mention the National Plant Board. The NPB focuses on managing plant pests (insects, pathogens, etc.) and invasive plants. The NPB recently celebrated its centennial anniversary. States have created fora under the NPB in which they exchange experiences with the goal of coordinating their efforts.

With respect to animal invaders (other than plant pests) or disease or parasite threats to animals, I believe there is no equivalent to the NPB. The Association of State Wildlife Agencies (AFWA) has an invasive species committee which discusses issues of general concern (see agenda from one of its meetings here).  This effort is much more recent than the NPB. It is similar in that it is consultative, with no authority to enforce a common approach.

Findings

Drake et al. (2026) explore the extent to which American states apply similar vs. different approaches to managing invasive species as a group and plants, invertebrates, and vertebrates separately. Lack of data forced them to exclude fungi and other microorganisms. They focused on 21 contiguous states in the eastern part of the country. They also compared the states’ lists of regulated species to national lists of invasive species compiled by the United States’ Register of Invasive and Introduced Species (US-RIIS) (Simpson et al., 2022; Simpson and Eyler, 2018) and U.S. Geological Survey Non-indigenous Aquatic Species database (NAS; U.S. Geological Survey, 2023).

A literature search revealed 1,117 state statutes, regulations, and similar policy documents that pertain to invasive species. One third of these documents (n = 448) named at least one taxon at the genus or species level. Of these, 35.3% named one or more plant species; 19.9% named one or more invertebrate; and 44.8% named vertebrates. Overall, 60.5% of these species were listed by only one state. Viewed by taxonomic group, this broke down to 40.6% of plant species, 60.6% of invertebrates, and 56.4% of vertebrates. Only four species are regulated in all 21 states = western (European) honeybee (Apis mellifera); and three agricultural weeds, creeping thistle (Cirsium arvense), quackgrass (Elymus repens), and dodder (Cuscuta species).
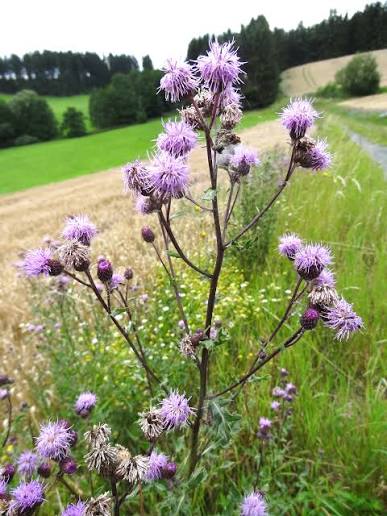
Cirsium arvense; photo by USchmidt via WikiMedia

Drake et al. (2026) found neighboring states did not share similar species lists or approaches. Consistency was even less at the regional scale, particularly when managing invasive invertebrates or vertebrates. The absence of a unified approach means that proactive states are susceptible to invasion from neighboring states which take a less vigorous stance. Since managing invasive species becomes more difficult and costly as the invasion progresses, undermining proactive policies undercuts efficiency.

Even when the national government does act, it lacks a unified approach. No federal legislation mandates a central authority to direct and implement IAS detection and response. The National Invasive Species Council (NISC), established by Executive Order 13112 in 1999, is supposed to provide high-level leadership to help overcome barriers to communication and promote collaboration among the several federal agencies bearing responsibility for various aspects of the issue. Authors, e.g., Reaser, Simpson, et al. (2020); Simberloff et al. (2020), say NISC’s effectiveness has been undermined by inconsistent funding and vacillating political support from policy-level leaders.

Drake et al. (2026) also assessed which of the 21 states took action proactively. Two plant species were listed by name by all 21 states: quackgrass (Elymus repens) and creeping thistle (Cirsium arvense). They called three states (14.3%) “pro-active” because they regulated quackgrass before it was detected in the state. Four states (19%) did the same regarding creeping thistle. The one invertebrate species listed by all 21 states, the western (European) honeybee, was established in these states before they began addressing invasive species, so it is not a test of states’ forethought.  

Of course, the policy goals differ between the two plant species and the honeybee: the former are considered damaging so policies focus on their control and management, whereas the honeybee is valued for pollination and honey production so policies aim at protecting it. There is no federal legislation regulating Apis mellifera individuals already in the country. State regulations governing interstate movement are the usual jumble of approaches. Drake et al. (2026) says this lack of consistency can increase the risk that introduced pathogens, pests, and undesirable subspecies (i.e., “Africanized” bees) will spread. They note that this chaos reigns despite bees’ importance to the agricultural sector.

Florida had policies governing the most species (345), Vermont the least (67). More surprising to me, New York regulated the most plant species (161); Mississippi the most invertebrates (105), and Virginia the most vertebrates (189).

Collectively the states regulate three times more species than appear on either national registry: 1,862 species in the state database versus 630 in US-RIIS or NAS databases. The states regulated a proportionally larger number of plant species and much smaller proportion of vertebrates. The number of species named in both state and federal databases were 360 plant species (57.1%), 170 invertebrates (28.4%), and 91 vertebrates (14.4%). The difference between federal and state lists is further magnified by the fact that significant numbers of species listed on the federal databases are managed by only one state: 143 plant species (48.3%), 86 invertebrates (29.1%), and 28 vertebrates (9.5%). In other words, only 217 plant species, 84 invertebrate species, and 63 of vertebrate species designated as invasive by federal databases were being managed by more than one state.
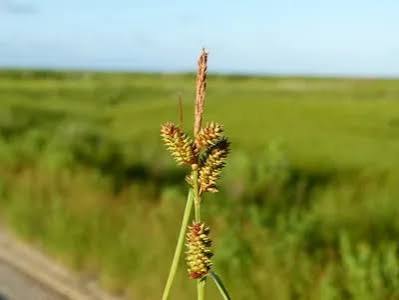
Carex extensa – one of plant species listed as invasive by USGS but not regulated by any of the 21 states; photo by botanygirl via Picture This

The survey identified a wide range of state agencies that have at least some responsibility for managing invasive species. These agencies’ principal concerns are agricultural, plant, or livestock industries; wildlife, fisheries, and recreation; forestry, mining, and natural resources; marine resources; public and environmental health; transportation, utilities, and commerce; and administration, education, specific locations, and all other types. Agriculture agencies are overwhelmingly responsible for invasive plants, insects, and arthropods; and almost equal to Fish and Wildlife departments in the case of managing molluscs. F&W departments are most often responsible for mammals, fish, crustaceans, amphibians and reptiles. Public and environmental health agencies are a distant second as regards responsibility for plants and arthropods, and third re: insects. Administration/education/specific location agencies are third most frequently given responsibility for plants; they hardly appear for other categories. Transport and commerce ranked fourth (nearly the same as public health agencies) for managing insects.

More than half of state policy measures (55.4%) related to terrestrial species, habitats, and pathways; 17.1% related to aquatic species, habitat, and introduction pathways; and 27.5% related to both.

Considering all species named in each state’s policy codes, about half of the listed taxa in each focal state’s policies are also listed by at least one neighboring state. At the regional level, overlapping or consistent policies declined to about 19% of the species. It doesn’t surprise me that New England states rank high in cooperation. Nor that the least number of species also regulated by neighboring states applies to Florida; the “sunshine state” is semitropical and has many types of ecosystems probably not present in Alabama or Georgia.

Once again, consistency is higher for plant species than the animal taxa. Among-neighbor overlap for plant taxa is ~69-70%, for invertebrates is ~50%, and for vertebrates only about a third. At the regional level, overlap is ~28% for plant species, ~18% for invertebrates, and 14% or less for vertebrates.
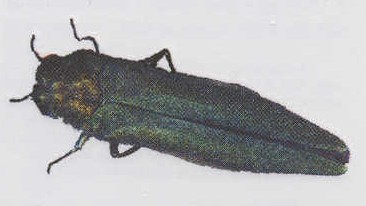
Drake et al. (2026) present case studies on several species to illustrate the breadth and depth of policy inconsistency, coordination, and implementation. The species studied are three of the four species regulated by all 21 states in the database; and three others selected to be emblematic of plant, invertebrate, and vertebrate taxonomic groups. The representative species for invertebrates is the emerald ash borer (EAB; Agrilus planipennis); the illustrative species for vertebrates is feral pigs (Sus scrofa). 

Drake et al. (2026) report that the EAB had been detected in all but two of the 21 states in their study – Florida and Mississippi (EAB has now been detected in the state). There was a federal quarantine until early 2021. Still, only 10 states (47.6%) have a policy regulating EAB per se. Nine states had acted proactively; this was the highest proportion among all the species analyzed, probably because the beetle spread so quickly and had such obvious and severe impacts observed.) My analysis of data on the Don’t Move Firewood website determined that few of these states regulate firewood. Seven states require treatment of firewood originating out-of-state. New York also prohibits movement of firewood within the state over distances exceeding 50 miles. Two states regulate firewood originating in location quarantined for a specific pest, e.g., EAB. Three states restrict movement of outside firewood onto state properties. The rest of the states urge people to “burn it where they buy it” but impose no requirements. In some cases, National parks for forests have more stringent regulations. I am quite disappointed how few states have taken protective actions. Drake et al. (2026) explained the absence of regulations in the other 11 states as possibly due to the slow pace of legislative action compared to the speed of spread. I think this factor deserves greater attention.

Drake et al. (2026) noted that there are cooperative programs that cross jurisdictional boundaries; these increase programs’ effectiveness. The example they cite is the Ash Protection Collaboration Across Wabanakik — a cooperative effort among federal, state, and tribal governments and non-governmental organizations in northern New England and bordering Canadian and tribal lands.

The discussion of feral pigs reported that these animals are becoming increasingly troublesome. The highest density of pig populations is in southern states but suitable habitat is found across North America. Twelve states have adopted relevant policies; five were proactive in doing so. Feral hogs are present in at least three of the nine states that lack any policy; they are also present in neighboring states of most. Drake et al. (2026) say that the patchwork of policies and regulatory agencies across (and even within states) has hindered management. One of the issues with feral hog management is the presence of conflicting views and stakeholders. Some states encourage hunting, others outlaw it in hopes of reducing any motivation to transport hogs to new areas to initiate sport hunting. They conclude that prohibiting private landowners from profiting from feral pig hunting opportunities, while apparently useful for control, might not be reasonable.

Drake et al. (2026) notes that there is no national policy but the federal government does provide financial assistance. Congressional legislation created the Feral Swine Eradication and Control Pilot Program (FSCP), co-managed by USDA Natural Resources Conservation Service and APHIS. They say that while federal and state investment is likely necessary to conduct the large-scale control needed, the public wants the opposite: they say those responsible for pig releases and individual landowners should pay for control efforts. Drake et al. (2026) discuss the situation in North Carolina to illustrate the conflicting approaches within one state.

Drake et al. (2026) find the greatest consistency across states in the regulation of invasive plants. This might reflect the historical attention to agricultural weeds. However, there are still inconsistencies that might cause confusion and facilitate unintended spread of invasive plants by the horticultural trade. (See my earlier blog here.) They point out that the lack of attention to invertebrates and vertebrates falls short considering the risks and costs these invaders impose at the national and global levels. In the eastern United State, five of the six costliest invasive species are invertebrates; the sixth is feral hogs.

Drake et al. (2026) worry that the widespread differences in approach leads to inaccurate estimates of invasive species’ economic cost as well as reduces states’ ability to effectively plan and coordinate efforts. They concede that given the range of agencies and industries that contribute to invasive species management, their review of state policies might not accurately reflect the full effort. Also the engagement of multiple players enhances flexibility. However, the disconnect between policy and on-the-ground actions can be a barrier to effective communication and compliance. It might also result in duplication and missed opportunities for collaborative management on common goals in neighboring states.

Drake et al. (2026) concede that social acceptance affects implementation. The most cost-effective, efficient, and impactful control methods might be socially unacceptable. Often social acceptance comes after an invasive species has spread and established – so after counter action is most successful and cost-effective.

Drake et al. (2026) note that climate change is likely to reduce barriers to invasive species’ spread and establishment and facilitate transition of benign non-indigenous species into damaging invaders. They say there is an urgent need for more attention from policymakers to the threat posed to both the economy and ecological systems. Their example is the contrast between the concentration of forest insect pests in the northeast while Florida and Mississippi list the highest number of species. Drake et al. (2026) suggest these listings reflect the region’s forestry sector’s concern about non-native pests – but I have not seen such interest (See profile of Sirex woodwasp here.)

To reduce vacillations in federal policy when administrations change, Drake et al. (2026) urge Congress to adopt strong, overarching legislation. If that isn’t possible, they say the second best option is to strengthen incentives and procedures for interstate cooperation. Such an approach could be extended to Canadian provinces

Drake et al. (2026) say it is clear from their own and others’ work that current policy tools fall short and leave proactive states at risk of threats from their neighbors. A possible model is competitive and non-competitive State Wildlife Grants program managed by the U.S. Fish and Wildlife Service. These funds should complement, not be reallocated from, current conservation efforts.

They praise some efforts by NISC, specifically the Early Detection Rapid Response framework, as a way to spur improved communication among policymakers, practitioners, and researchers. However, given the many remaining legislative and regulatory gaps, and differing interpretations, they suggest increasing opportunities of practitioners to use existing research and outreach structures e.g., Land Grant institution extension model. New frameworks such as translational invasion ecology can improve identification of research priorities and transfer of generated knowledge. These frameworks explicitly take into account the ecological, sociological, economic, and political contexts. Incorporating diverse stakeholders and quantitative tools e.g., through simulations, climate change projections, connectivity assessments, and species distribution maps that take into account the socio-economic components might be able to more holistically evaluate and act upon the potential threats.

Drake et al. (2026) call for increased attention to researching species likely to become problematic in the future. They note that only four of 18 NIS species in New England identified by another’s study as likely to benefit from climate change are included under policies of at least one state in the region.

SOURCE

Drake, J., E.M.X. Reed, D. Haak, B. Brown, M.C. Mims, M.G. Sorice, H. Rogers, S. Salom, T. Schenk, and J.N. Barney. 2026. State Lines and Species Divides: Inconsistencies and Opportunities in Invasive Species Policies across the eastern United States. Ecological Applications 36(5): e70287. https://doi.org/10.1002/eap.70287

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Ash in the East: Can the many seelings & saplings reach reproductive age?

EAB-caused mortality of ash in Midwest; photo by Nathan Siegert, USFS

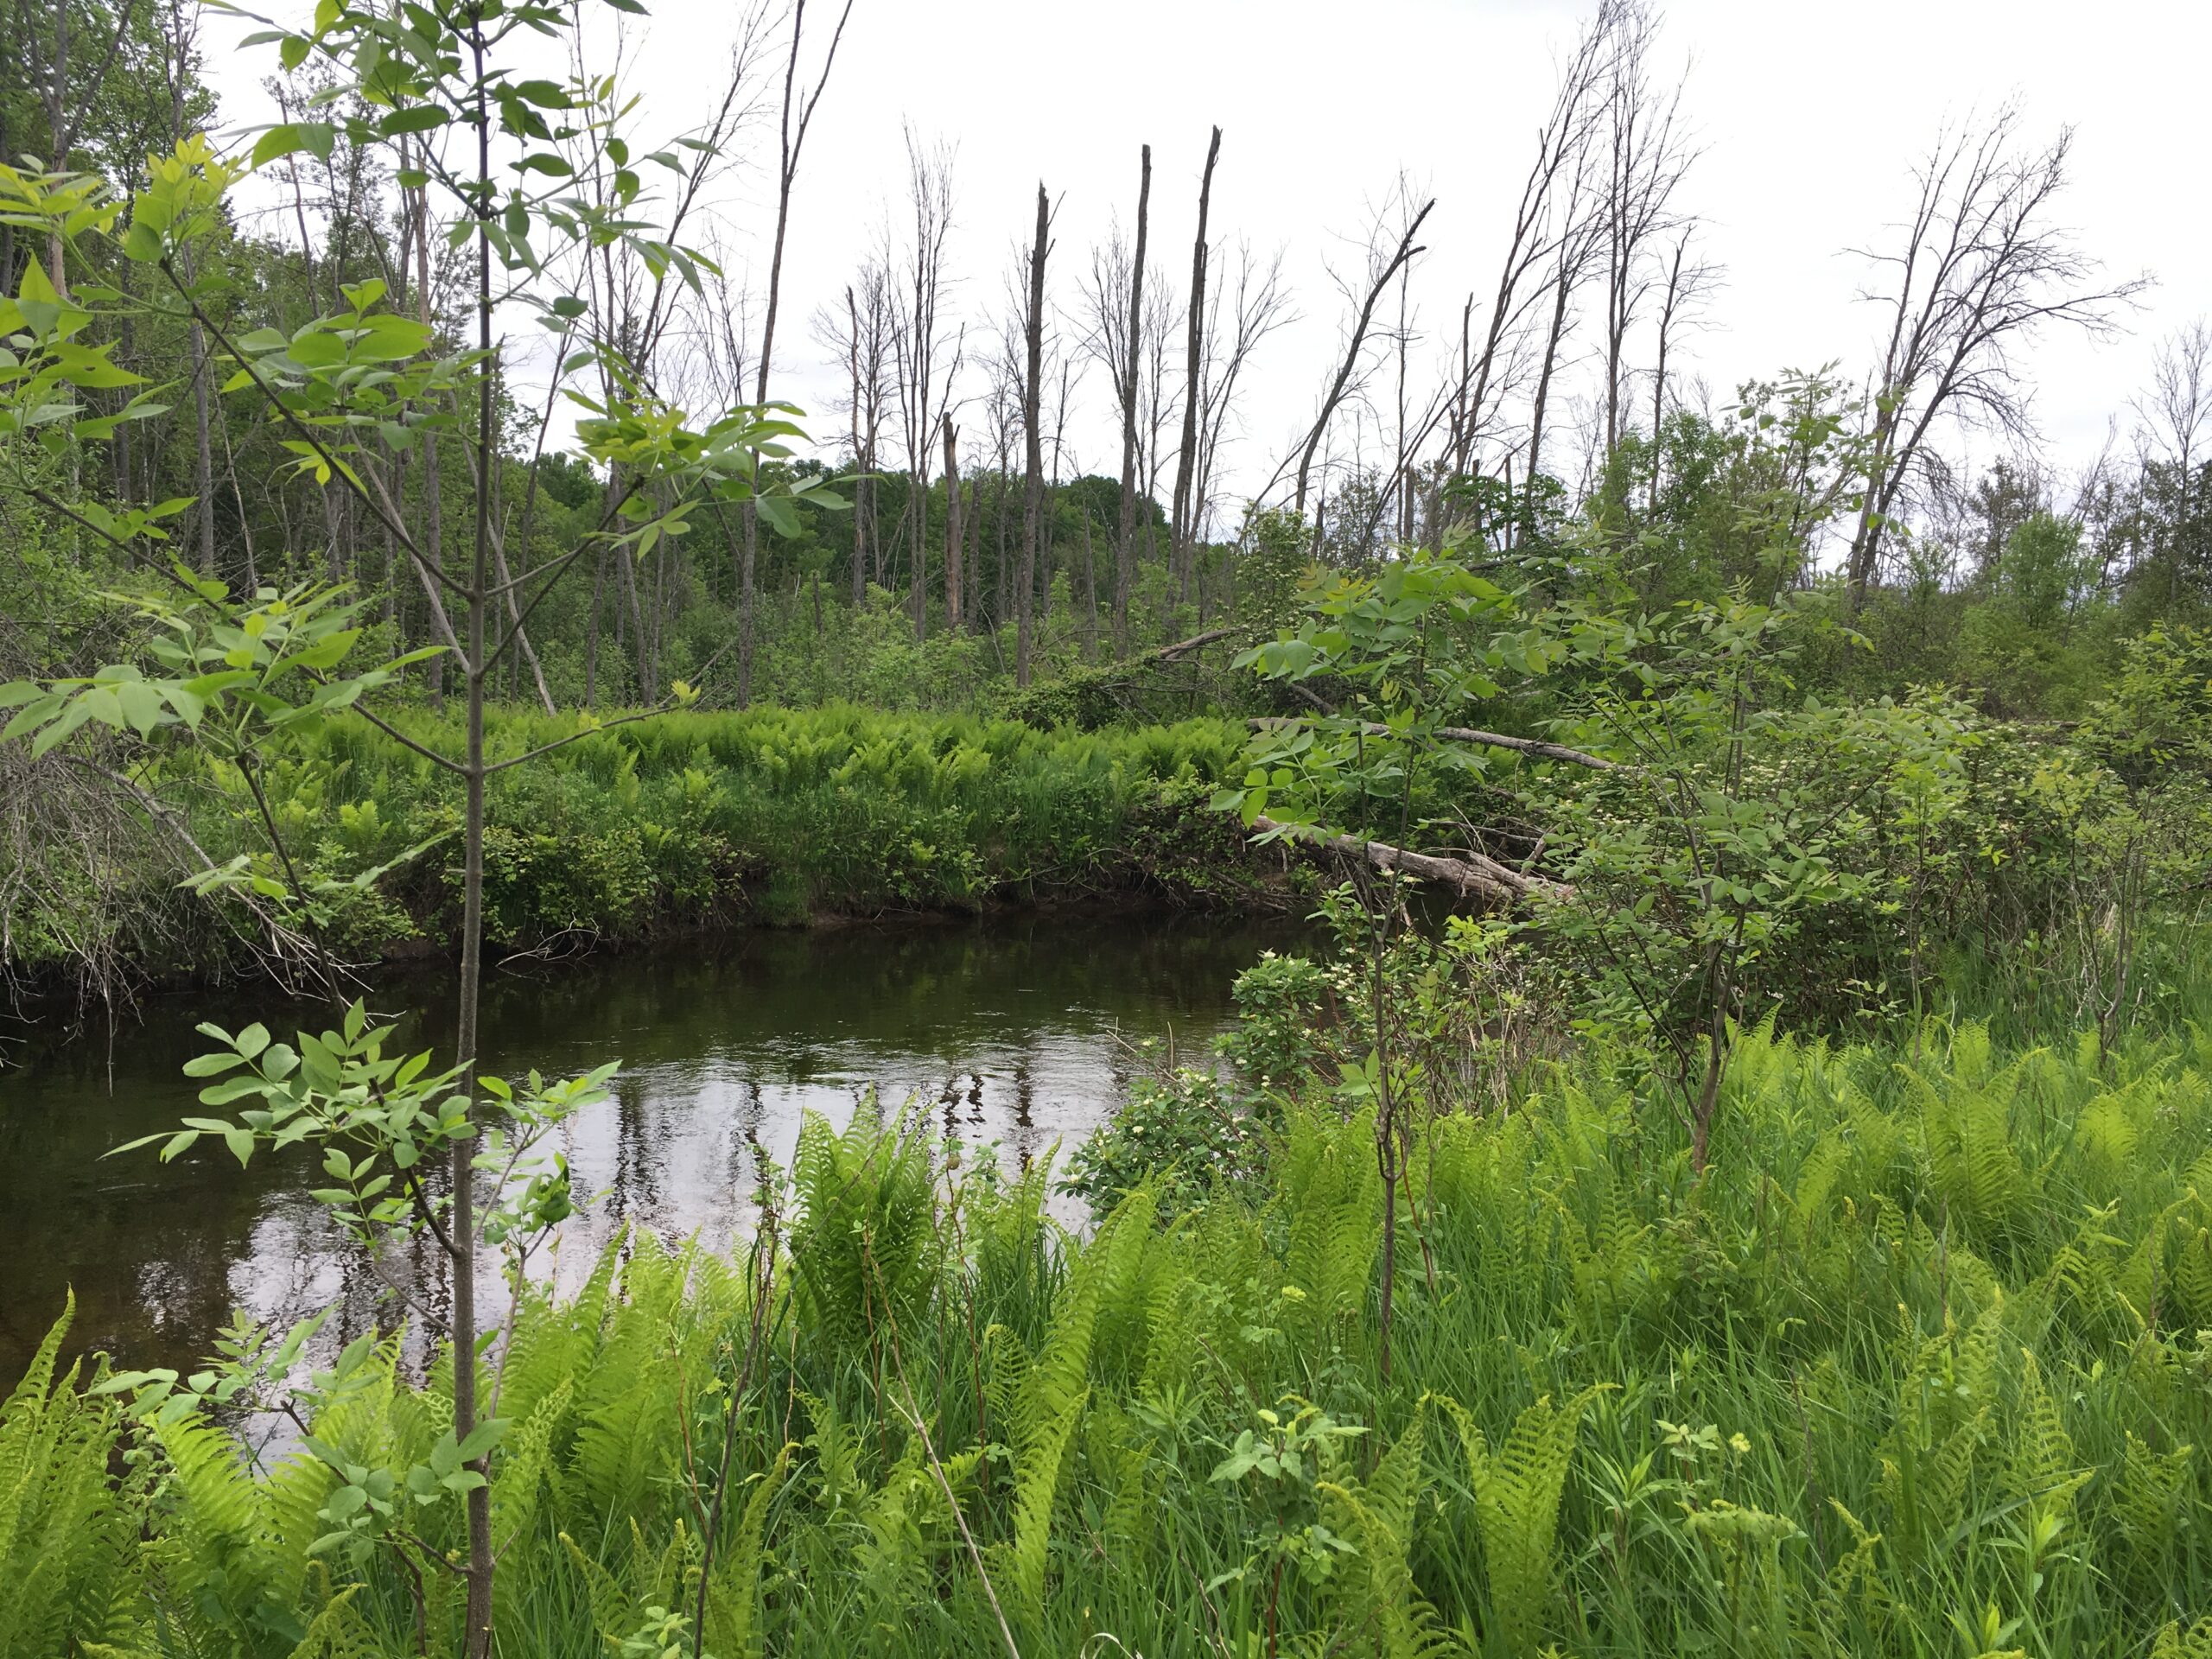
The 20th anniversary of detection of the emerald ash borer (EAB; Agrilus planipennis) in southeast Michigan has prompted reviews of the current situation. Tayal and Perry (2026) analyzed data from invasion-spanning research sites to investigate the extent of ash regeneration. Mortality of black ash (Fraxinus nigra), green ash (Fraxinus pennsylvanica), and white ash (Fraxinus americana) had exceeded 99% in these forests, with a concurrent precipitous decline of viable seed production.

They found that regenerating ash are abundant in the understory of post-outbreak forests. Among the 638 understory trees in the survey, basal area was highest for ash, followed by elm (Ulmus species.), maple (Acer species.), and musclewood (Carpinus caroliniana). On upland (xeric) and riparian (mesic) sites, ash are primarily in seedling and sapling size classes. Larger ash are more plentiful in wetland forests; the seven canopy ash trees were all in wetland forests.

The emerald ash borer is present in low numbers in all study sites.

Many ash of susceptible size (≥2.5 cm dbh) have symptoms of EAB infestation. Several of these symptoms (e.g., woodpecker damage, presence of epicormic sprouts, and canopy decline) grow more established as the trees grow. Still, 57% trees ≥5 cm dbh have healthy canopies. D-shaped adult beetle exit holes were detected on only 2% of the ash.

black ash swamp in Minnesota; photo by Eli Sagor via Flickr

Tayal and Perry (2026) concluded that the black and green ash in wetland forests are able to respond quickly to the multi-tree gaps produced by EAB-induced death of their dominant predecessors in these systems. These gaps result in more light availability and growing space than the single-tree gaps created by mortality of individual ash in mixed-species riparian or upland systems.

Other tree species that also flourished in the aftermath forests were maples, esp silver maple (Acer saccharinum), have become dominant in the overstories of wetland forests in northern US and Canada. In late successional floodplain forest systems, the maples are joined by other species with a tolerance for cold, flooding, and shade including elm (e.g., Ulmus americana); tamarack (Larix laricina) and yellow birch (Betula alleghaniensis).

Of course, American elm is threatened by a separate invasive species, the pathogens Ophiostoma ulmi and O. novo-ulmi. 

Tayal and Perry (2026) state several times that the future survival of this “orphaned” cohort of seedlings and saplings too small to have been colonized by EAB during the initial outbreak is uncertain. As they grow to susceptible size will they be attacked and killed by a growing population of beetles? Or will the biocontrol agents – assisted by woodpeckers – be effective in keeping EAB populations sufficiently low to allow the immature ash to reach reproductive size? Tayal and Perry (2026) cite Duan et al. (2023) as reporting that there is some evidence that the biocontrol agents can suppress EAB densities in immature ash. [Three agents – Oobius agrili, Spathius galinae, and Tetrastichus planipennisi – are established – in low numbers – in the forest sites studied.] So while the extent to which BC agents have protected regenerating ash in these long-term plots is still unknown, they express the hope that the parasitoids might be most effective in aftermath forests after EAB populations have peaked and then declined.

SOURCE

Tayal, A. and K.I. Perry. 2026. Status of ash (Fraxinus species.) in mixed hardwood post-outbreak forests near the epicentre of the emerald ash borer invasion. Agricultural and Forest Entomology, 1–12. Available from: https://doi.org/10.1111/afe.70067

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

EAB in Pacific Northwest: likely impacts (expanded)

the Oregon ash-dominated wetland in Arkany National Wildlife Refuge in Oregon’s Willamette Valley; photo by Wyatt Williams, Oregon Department of Forestry

Two years ago I posted a blog summarizing the probable impact of the emerald ash borer (EAB; Agrilus planipennis) in Oregon. Reminder: the EAB was detected in Forest Grove, Oregon (west of Portland) in 2022. Scientists determined that it had been present for four to six years at that time.

In her Master’s thesis, Chloe Hull (2024) confirms that nearly all forested wetlands in the state’s Willamette Valley are comprised overwhelmingly of Oregon ash (Fraxinus latifolia). Therefore, these wetlands are likely to undergo rapid, significant shifts in vegetation, hydrology, and soils — unraveling their ecosystem functions. Hull warns that no management approach can restore those wetlands to perform the full breadth of their pre-settlement function and diversity. She suggests instead strategies to maintain these areas as wetlands – even if different types.

Hull’s conclusions are based on the expectation that Oregon ash will be killed by EAB infestation at levels similar to black (Fraxinus nigra), white (F. americana), and green (F. pennsylvanica) ash in the Midwest, i.e., up to 99%.

What is Threatened?

Wetlands provide numerous benefits to both human and natural systems, including purification of surface waters, habitats for plant and animal species, and food sources. Hull cites studies estimating that natural wetlands deliver 43.5% of the total global monetary value of ecosystem services provided by all natural biomes despite making up only ~3% of the world’s surface area.

In the Lower 48 United States more than half of wetlands have been converted to other land use types since 1780. In Oregon statewide, the extent of loss is lower: 38%. However, in the Willamette Valley specifically, the estimated loss is 57%.

Hull describes the pre-settlement wetlands of the Willamette Valley and the forces that have transformed them.

The most widespread of these wetlands were wet prairies, covering about 137,277 ha. Wetland, or bottomland, forests occupied about 97,477 ha. These forests typically formed bands along river or stream channels; they were also found occasionally in beaver swamps. These forests were composed of fire-intolerant deciduous trees in various densities. Stands along active channels typically willows (Salix species.), red alder (Alnus rubra), white alder (Alnus rhombifolia), and black cottonwood (Populus trichocarpa). On slightly higher terraces, where the inundations were less frequent, grew Oregon ash, bigleaf maple (Acer macrophyllum), and Oregon white oak (Quercus garryana). Ash and oak were particularly important along many smaller stream channels surrounded by open prairies.

Kinkaid’s lupine; photo from “Picture This” website

The wet prairies provide habitat for two federally-listed endangered plant species [Willamette daisy (Erigeron decumbens var. decumbens) and Kincaid’s lupine (T. Lupinus sulphureus species. kincaidii)]; and four state-listed species [white rock larkspur (Delphinium leucophaeum), peacock larkspur (Delphinium pavonaceum), Willamette navarretia (Navarretia willamettensis) and white fairy poppy (Meconella oregana)].  Two plant species and a butterfly formerly listed by the U.S. Fish and Wildlife Service [golden paintbrush (Castilleja levisecta) and Bradshaw’s lomatium (Lomatium bradshawii), and the Nelson’s checkermallow (Sidalcea nelsoniana)] are also present.

Both types of wetlands were maintained in part by periodic burning by the resident Indigenous peoples. These actions promoted a habitat mosaic of tufted hairgrass (Deschampsia cespitosa) prairies, camas lily (Camassia quamash) wet prairies, Oregon white oak savannas, and ash-dominated bottomland riparian forests. The Willamette River meandered and formed braided channels, with resulting flooding and wetland habitats.

In 1855 the federal government forced the Indigenous peoples to leave the valley. Since then, the wetlands have been drained and converted into agricultural fields; or drowned by various flood-control dams, diversions, and levees. As a result, Hull says, the Willamette Valley has been largely disconnected from the river. In addition, Euro-Americans have introduced non-native plants and intensive livestock grazing. Overall, the valley has lost the wetlands’ ecosystem functions.

Current (pre-EAB-induced mortality) Context

In the absence of disturbance, ash tends to be most important early-seral and final climax tree species. It plays a crucial role in regulating and supporting other species, hydrology, carbon storage, nutrient cycling, and overall resource availability.

Oregon ash are medium-sized trees, growing up to 24 m (80 ft) high and a dbh of 75 cm (30 in). Ash are long-lived, probably up to 250 years. They are thought to reach sexual maturity at ~ 30 years.

Oregon ash are adapted to the clayey, soggy conditions of the valley. (The average clay component of Willamette soils is 60-70%. When they become saturated there is prolonged surface ponding.) They also occupy drier, well-drained sites. Ashes’ tolerance of other environmental conditions, e.g., flooding, drought, salinity, soil pH, etc., is unknown.

Hull based her conclusions on analysis of four ash-dominated wetlands in the central Willamette Valley. Although only ~ 24 km apart, the sites differ in vegetation community composition, hydrology, and past and current other management goals.   

Site number 1 (Jackson Frazier) comprises primarily wetlands; current management is attempting to restore the wet prairie system, with little attention to forested wetlands. The second site (Mulkey Creek) is managed primarily to maintain oak woodland and prairie habitat. The third site (Poultry Center) is a university research facility. The fourth site (Shedd) has both natural drainage (two sloughs and a creek) and a relatively intact bottomland forest. This property often hosts public off-roading events so owners maintain trails and camping areas.

Hull determined vegetation types and management activities on these sites since 1948 by examining aerial photographs.

At all sites ash trees grew larger and stands increased in density between 1948 and 1978. Averaged across all sites, Oregon ash comprise more than 92% of forest canopy composition. The species reached 100% in some plots at some of the four sites. The second most common species in the canopy is the native black hawthorn (Crataegus douglasii). Among the other species are several non-native fruit or flowering trees [crabapple (Malus species.), pear (Pyrus species.), plum (Prunus species.)], Oregon white oak, and other species. Overall ash density was highest in the Shedd site, decreasing through Poultry Center and Mulkey Creek to Jackson Frasier. Rankings were different when she considered the balance between adult and sapling ashes: Jackson Frasier has the highest proportion of ash seedlings (93% of total saplings at one plot; 75% at a second); Poultry Center ranked second (70% of all saplings across all study quadrants). There are very few ash saplings at Mulkey Creek and Shedd (the last has only 4 ash saplings on the entire study site). Hull attributes these very low numbers to competition between adult and sapling ash.

EAB damage along a Mid-Atlantic river; is this what will happen in Oregon? photo by Leslie A. Brice

Anticipated Impacts of Ash Mortality

Hull expects 99% mortality of ash trees across the Willamette Valley in eight to 15 years. This will cause complete restructuring of the forest canopy and subsequent changes in disturbance regimes, flora and fauna communities, and land use. Currently there is no feasible way to restore ash-dominated wetlands. She explored three alternative future states, one of which describes several possibilities for maintaining different wetland ecosystem types.

Noting experience in the East, Hull concludes that there is extremely limited potential for ash regeneration following EAB-induced mortality. In the East an “orphaned cohort” of ash trees too small to have been infested in the initial invasion, or which sprouted after that event, has persisted so far. But its long-term survival and maturity is uncertain because EAB remain. See non-PMW article Especially since Oregon ash does not reach reproductive age for 30 years), tree mortality is likely to exceed seedling recruitment in these stands.

Still, since ash seeds banks decline rapidly after adult trees die, the orphaned cohort remains the most realistic opportunity for ash regeneration. It is hoped native woodpecker species and introduced biocontrol agents can sufficiently suppress EAB populations to create an opportunity for the saplings to achieve maturity and reproduce. See non-PMW article

Restoration

A majority of the literature and information about EAB effects on ash wetlands is from the Midwest. Willamette wetlands differ in soil characteristics and biotic and abiotic ecosystem components. Unlike the moderate to deep organic histosols underlain by clay in the Midwest, Willamette soils are hydric, defined as “a soil that formed under conditions of saturation, flooding, or ponding long enough during the growing season to develop anaerobic conditions in the upper part”. As noted above, saturation of these soils often results in prolonged surface ponding. Another factor is that most of the precipitation in Oregon is rain, not the snow of the upper Midwest. 

Hull evaluates the probability of maintaining each of her four sites as a wetland. She also considers how to prevent domination of the site by either currently established or newly introduced invasive weed species.   

Research in the Midwest indicates that wetland vegetation – in that case especially black ash trees — has a large influence on water table levels throughout the growing season. Simulated ash mortality led to a significant reduction in evapotranspiration and drawdown rates and a long-term rise in the water table. This was expected to promote conversion to open (herb-dominated) or shrub-dominated marshes.

In the Willamette Valley there are two types of wetlands not dependent on tall-stature trees – which are likely to disappear.

restored wet prairie near Eugene; photo by Bureau of Land Management

Pre-settlement, Willamette Valley wetlands were primarily wet prairies. Even now similar wetlands exist; they support a wide diversity of perennial and annual forbs and graminoids. Their floral diversity is due partly to traditional burning, partly to fine-scale vertical structures (“pedestals”) three to 20 cm high that support grasses and forbs on higher portions, rushes, sedges, and annual forbs on the lower, more often inundated surfaces. 

The second type of non-forested wetland is Scrub-Shrub Wetland. These occupy an ecological niche between a wet prairie and a forested wetland. They are dominated by fire intolerant woody vegetation kept short in stature by environmental conditions. Hull reports that these are relatively stable systems. They were once commonly maintained by beavers; Hull does not speculate about possibly restoring those ecosystem engineers. She does consider them to be potentially a successional stage in transition toward a forested wetland system. Oregon white oaks are among full-stature trees that can grow in these wetlands – in shrubby form.

Is it possible to restore forested wetlands by planting tree species other than ash? The success of this approach is challenged by the high clay component of soils and high water tables. None of tree species commonly associated with Oregon ash (red alder, black cottonwood, and bigleaf maple) can tolerate the same high clay soils. The species that do grow in clay soils (black hawthorn, some willows) are small (typically less than 6 meters tall) so they cannot fill the same ecological functions and niches as ash. A few large-form trees might tolerate saturated clay soils and serve a more similar ecological role. Hull names Oregon white oak and Willamette Valley ponderosa pine (Pinus ponderosa var. willamettensis). But these species are less tolerant of inundation.

Oregon white oak; photo by born1945 via Flickr

I notice the importance of Oregon oak (Quercus garryana) – both in existing forest and scrub habitats and as a possible replacement for ash. I am concerned that Hull does not mention that Oregon oak is also threatened by a non-native insect, the Mediterranean oak borer (Xyleborus monographus). Given this species’ presence I doubt that Oregon oak is a viable species for restoration of wetlands. I hope other scientists are exploring strategies for minimizing MOB’s damage to this important species.

Hull also discusses some tree species from elsewhere that are reported to be under consideration for planting in Willamette Valley wetlands. Several of these also are vulnerable to established non-native insects or pathogens. These include:

  • California black oak (Quercus kelloggii) – vulnerable to both the sudden oak death pathogen (Phytophthora ramorum) and the goldspotted oak borer (Agrilus auroguttatus). The latter is not yet found in Oregon.
  • Oregon myrtle (Umbellularia californica) – a host that supports sporulation by the sudden oak death pathogen (Phytophthora ramorum). SOD is established and spreading in southwest Oregon, on the other side of the coastal mountain range from the Willamette Valley.
  • Fremont cottonwood (Populus fremontii) and boxelder (Acer negundo) — both are vulnerable to yet other non-native beetles, the Euwallacea-fungus complex known in California as “invasive shot hole borers”. The closest known population of the complex is in the San Francisco Bay area.

Hull notes that in the Midwest, scientists are considering several species as potential replacements for black ash, including American elm (Ulmus americana), swamp white oak (Quercus bicolor), red maple (Acer rubrum), eastern white-cedar (Thuja occidentalis), and common hackberry (Celtis occidentalis). In this case she mentions concern around the viability of American elm in the presence of “Dutch” elm disease. The disease is present on elms planted in Portland and possibly other cities in Oregon.

Hull notes that little research has been conducted on questions now considered important, such as the ecological functioning of forested wetlands – including those in the Willamette Valley – and vegetation responses to changing water tables. As she points out, during the time it will take to assess replacement trees ash will probably be extirpated.

The Threat from Invasive Plants

Hull reports the presence of several state-designated noxious weeds in the Willamette Valley that pose a threat to maintaining natural wetlands. The two most common and persistent weeds in the valley’s wetlands are Himalayan blackberry (Rubus armeniacus) and reed canary grass (Phalaris arundinacea). She names several other species, including lesser celandine (Ficaria verna/Ranunculus ficaria) and Japanese knotweed (Polygonum cuspidatum) (both are highly invasive Mid-Atlantic bottomlands); several trees and shrubs; and various grasses.  

Ficaria invasion in the Mid-Atlantic; photo by F.T. Campbell

Management Options

Considering management options, Hull thinks it unlikely that officials will decide to do nothing because forests of standing dead ash are dangerous. She believes the best option is to harvest 20% of ash stands in 0.04 ha gaps and promote woody shrub establishment. Shrubs can provide some shade to streams and continued evapotranspiration and offset large rises in water table levels. The large amounts of down woody debris in streams could increase stream complexity and habitat as well as mitigate channelization. Hull notes that the resulting scrub-shrub habitats were common pre-settlement.

Regarding her four study sites, Hull considers two (Mulkey Creek and Shedd) are likely to become scrub-shrub wetland communities. Opportunity to plant tree seedlings at Shedd will depend on the density of understory vegetation. A third site, Poultry Center could transition to either an emergent (herb-dominated wetland or a scrub-shrub community. The direction of changedepends on whether increased surface evaporation leads to less ponding; or reductions in evapotranspiration rates leads to more ponding. Poultry Center is a reasonable candidate for tree species substitution if the hydrologic shifts are favorable. The wettest site, Jackson Frazier, will probably become an emergent wetland community, with a higher water table. It offers limited opportunities to establish alternative tree species.

Management of wetlands is further constrained by multiple restrictions, including state and federal laws; funding limitations; and visitor perceptions.

SOURCE

Hull, C. 2024. A Valley Without Ash: Exploring Strategies for Forested Wetland Restoration Post Emerald Ash Borer Invasion in the Willamette Valley, Oregon. MS thesis submitted to Oregon State University for the degree of Master of Forestry in Forest Ecosystems and Society

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

EAB detected in Washington State; Pacific Coast states taking action

A newsletter issued by the Oregon Department of Forestry reports lots of action in Oregon and Washington in response to the presence of emerald ash borer (EAB; Agrilus planipennis). (To subscribe to the newsletter, email Jim Gersbach at jim.gersbach@odf.oregon.gov)

Ash-dominated swamp in the Willamette Valley; photo by Wyatt Williams, Oregon Department of Forestry

In Oregon, where EAB was detected in 2022, cities are taking protective actions. In Portland EAB was officially detected inside city limits in late summer 2025 east of the I-205 freeway. So far the beetle has not been reported from elsewhere inside city limits. To better establish where EAB is present, officials plan to girdle 4 ash trees in spring 2027 in hopes that female EAB will be attracted to them and oviposit. Those trees will be cut down in the fall, then examined to determine if any larvae are inside. This method has been used to help pinpoint where EAB is spreading before obvious signs of tree dieback are apparent. Oregon Department of Forestry will demonstrate the techniques for staff from the City of Portland, Oregon Dept. of Agriculture, U.S. Forest Service, Washington Dept. of Natural Resources, and Clackamas Soil & Water Conservation District.

EAB was confirmed within the city limits of Beaverton during summer 2026. The Beaverton City Council has adopted legislation expanding pesticide protection to1,400 ash street treesabove the 600 already treated in 2025. Treatment – injection of emamectin benzoate – is scheduled to begin in spring 2027 and be completed by September 2027. Last year city workers also protected 22 significant native Oregon ash trees (Fraxinus latifolia) over 20” dbh in a city-maintained natural grove that is predominantly ash.

EAB was detected in Silverton by a local tree care professional in summer 2026. The nearby Oregon Garden responded by treating eight ash trees on its grounds – all exotic to the region (seven white ash [eastern North America] & one narrow-leaved ash [Europe]). The Garden receives ~100,000 visitors a year.  The treatments were supervised by Oregon Dept. of Forestry & Oregon Forestry Resource Institute staff.

In Washington State, where EAB was detected in August 2026, near Vancouver, the state has regulated firewood imported from sources outside the state. The quarantine on untreated firewood from outside the state was adopted in February by the state Legislature. It took effect on August 18.  The rule prohibits importation into WA of untreated firewood from outside the state. Firewood imported into WA must be heat-treated to a minimum woodcore temperature of 160o F (71o C) for at least 60 minutes or receive an equivalent WSDA-approved treatment. The wood must also be labeled to show its source & display the statement “Approved Pest Free”. Firewood harvested within Washington State is exempt as are processed wood products, such as compressed wood bricks, wood pellets, logs, or wood products transported for industrial uses, such as to sawmills, pulp & paper mills, & biomass or wood composite facilities. Civil penalties up to $5,000 per violation can be imposed.

The newsletter provides updates on Europe’s double threat: EAB & ash dieback pathogen. 

Europe is home to three species of ash: common ash (Fraxinus excelsior), manna ash (F. ornus), & narrow-leaved ash (F. angustifolia). 

Hungary is the first European Union country with a confirmed EAB infestation (summer 2026). Neighboring Slovakia has also reported EAB presence but this is still unconfirmed.  

While the EAB is native to the Russian Far East & other parts of East Asia, it was not seen west of the Ural Mountains before 2007, when it was reported in western Russia. By 2019 the pest had been recorded in Ukraine & Belarus. Researchers at Ohio State University have found that F. excelsior has at least moderate resistance to EAB.

Fraxinus excelsior in Belgium; photo by Jean-Pol Gramont

The ash decline pathogen (Hymenoscyphus fraxineus) is also from East Asia. It was first described in Poland in 1992 [although probably present much earlier, perhaps the 1990s (Tolio et al., 2025)]. It is now widespread in Europe. Where present, it has killed the vast majority of ash trees. To ascertain whether Oregon ash (Fraxinus latifolia) might be attacked, USDA Forest Geneticist Richard Sniezko of the Dorena Genetic Resource Center has sent seed to European colleagues so that they can plant them and track the results.   

Some good news: British scientists report ~5% of F. excelsior trees appear to exhibit resistance to the parthogen and in some ash groves in northern England ~90% of young seedlings appear to be resistant.

The USDA Forest Service will hold a webinar on Oct. 6th to discuss EAB resistance ash breeding 

Mary Mason, a geneticist w/ USFS Northern Research Station, will present. The webinar starts at 1 PM Eastern Daylight Time on Tuesday, Oct. 6.

Publications named by the Oregon newsletter that are particularly related to the situation in Oregon):

• Hull, C. 2024. A Valley Without Ash: Exploring Strategies for Forested Wetland Restoration Post Emerald Ash Borer Invasion in the Willamette Valley, Oregon. Oregon State University. https://ir.library.ORstate.edu/concern/graduate_projects/3j333b36w

• Melton, A.E., Faske, T.M., Sniezko, R.A., Thibault, T., Williams, W., Parchman, T. & Hamilton, J.A. 2025. Genomics-Driven Monitoring of Fraxinus latifolia (Oregon Ash) to Inform Conservation & emerald ash borer Resistance Breeding. Molecular Ecology e17640. https://doi.org/10.1111/mec.17640  

 • Monitoring Oregon ash forests in the face of the emerald ash borer: A guide for small woodland owners & managers https://extension.ORstate.edu/catalog/pub/em-9451-monitoring-OR-ash-forests-face-emerald-ashborer

• Larval development & parasitism of emerald ash borer (Agrilus planipennis) in Oregon ash (Fraxinus latifolia) & European olive (Olea europaea): implications for the West Coast invasion Journal of Economic Entomology | Oxford Academic

• Maze, D., Bond, J. & Mattsson, M. 2024. Modelling impacts to water quality in salmonid-bearing waterways following the introduction of emerald ash borer in the Pacific Northwest, USA. Biol Invasions (2024). https://doi.org/10.1007/s10530-024-03340-3  

• Kral, G. & D.C. Shaw. 2023. Alternatives to Ash in Western Oregon: With a Critical Tree Under Threat, These Options Can Help Fill Habitat Niche. Oregon State University Extension EM 9396. https://catalog.extension.ORstate.edu/em9396

• Oregon Ash: Insects, Pathogens & Tree Health by Oregon State University Extension (also available in Spanish)  https://extension.ORstate.edu/pub/em-9380  

Useful links for more information

Map to find where EAB is currently confirmed in Oregon: https://experience.arcgis.com/experience/9f29b1860cb04d36ad71b122148277f3

EAB monitoring guidance https://www.OR.gov/odf/forestbenefits/Documents/eab-monitoring-guidance.pdf

Oregon Department of Agriculture https://www.oda.direct/EAB  

Oregon Department of Forestry  https://www.OR.gov/odf/forestbenefits/pages/foresthealth.aspx  

Oregon State University Extension https://extension.ORstate.edu/collection/emerald-ash-borer-resources  

Emerald Ash Borer Information Network, a collaborative effort by the USDA Forest Service & Michigan State University www.emeraldashborer.info  

SOURCE

Tolio, B., P. Sherwood, D. Marčiulynienė, C. Crocoll, M. Cleary, M. Liziniewicz. 2026. Constitutive Metabolite Profiling of European & Asian Fraxinus with Varying Susceptibility to Ash Dieback. Journal of Chemical Ecology 52:8 https://doi.org/10.1007/s10886-025-01678-z

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Bioinvaders on Puerto Rico: More Complete Information

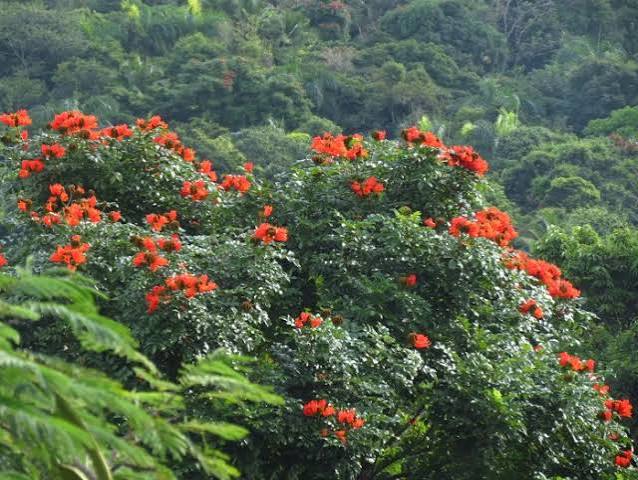
Spathodea campanulata (one of the most common invasive plant species in moist or wet forests on Puerto Rico); photo by Annika Lindqvist via EasyScape

America’s Caribbean islands have received much less attention that Hawai`i with regard to either their biological importance or level of biological invasion. I posted a blog three years ago about invasive tree species. I rejoice that the silence might be starting to change – thanks in large part to Julissa Rojas-Sandoval.

The West Indies

The Caribbean islands – including but not limited to Puerto Rico and the U.S. Virgin Islands – are considered one of 35 global BD hotspots on Earth (Castro, Quinones, and Gould 2016; Zimmerman et al. 2021). The most comprehensive descriptions are a decade old. Castro, Quinones, and Gould (2016) report that the Caribbean islands are home to ~14,526 plant and terrestrial vertebrate species, half of which are endemic to the region. At that time more than 900 species were on the IUCN Red List. The West Indies are characterized by exceptionally high levels of plant endemism, with more than 70% of seed plants considered endemic to the region (Rojas-Sandoval et al. 2017, citing earlier floristic assessments).

The Caribbean islands have a long history of anthropogenic disturbance – especially since Europeans arrived in 1492 — and intentional or accidental introductions of non-native species. Available sources differ on the number of species that should be categorized as “invasive”.

Potter et al. (2022) report that 17% of the flora of the islands of the Caribbean archipelago are not native. Rojas-Sandoval et al. (2017) identified 516 invasive non-indigenous plant species, representing about 4% of the total West Indian flora, and concluded that the incidence of invasive plants in the region is high compared with other island groups. Interestingly, each island group has its own suite of invasive species. More than 60% of these taxa occur on a single island. Thirty-eight percent belong to one of three families — Fabaceae, Poaceae, and Asteraceae. Thirty-four families are represented by a single species; 78 families by fewer than five.

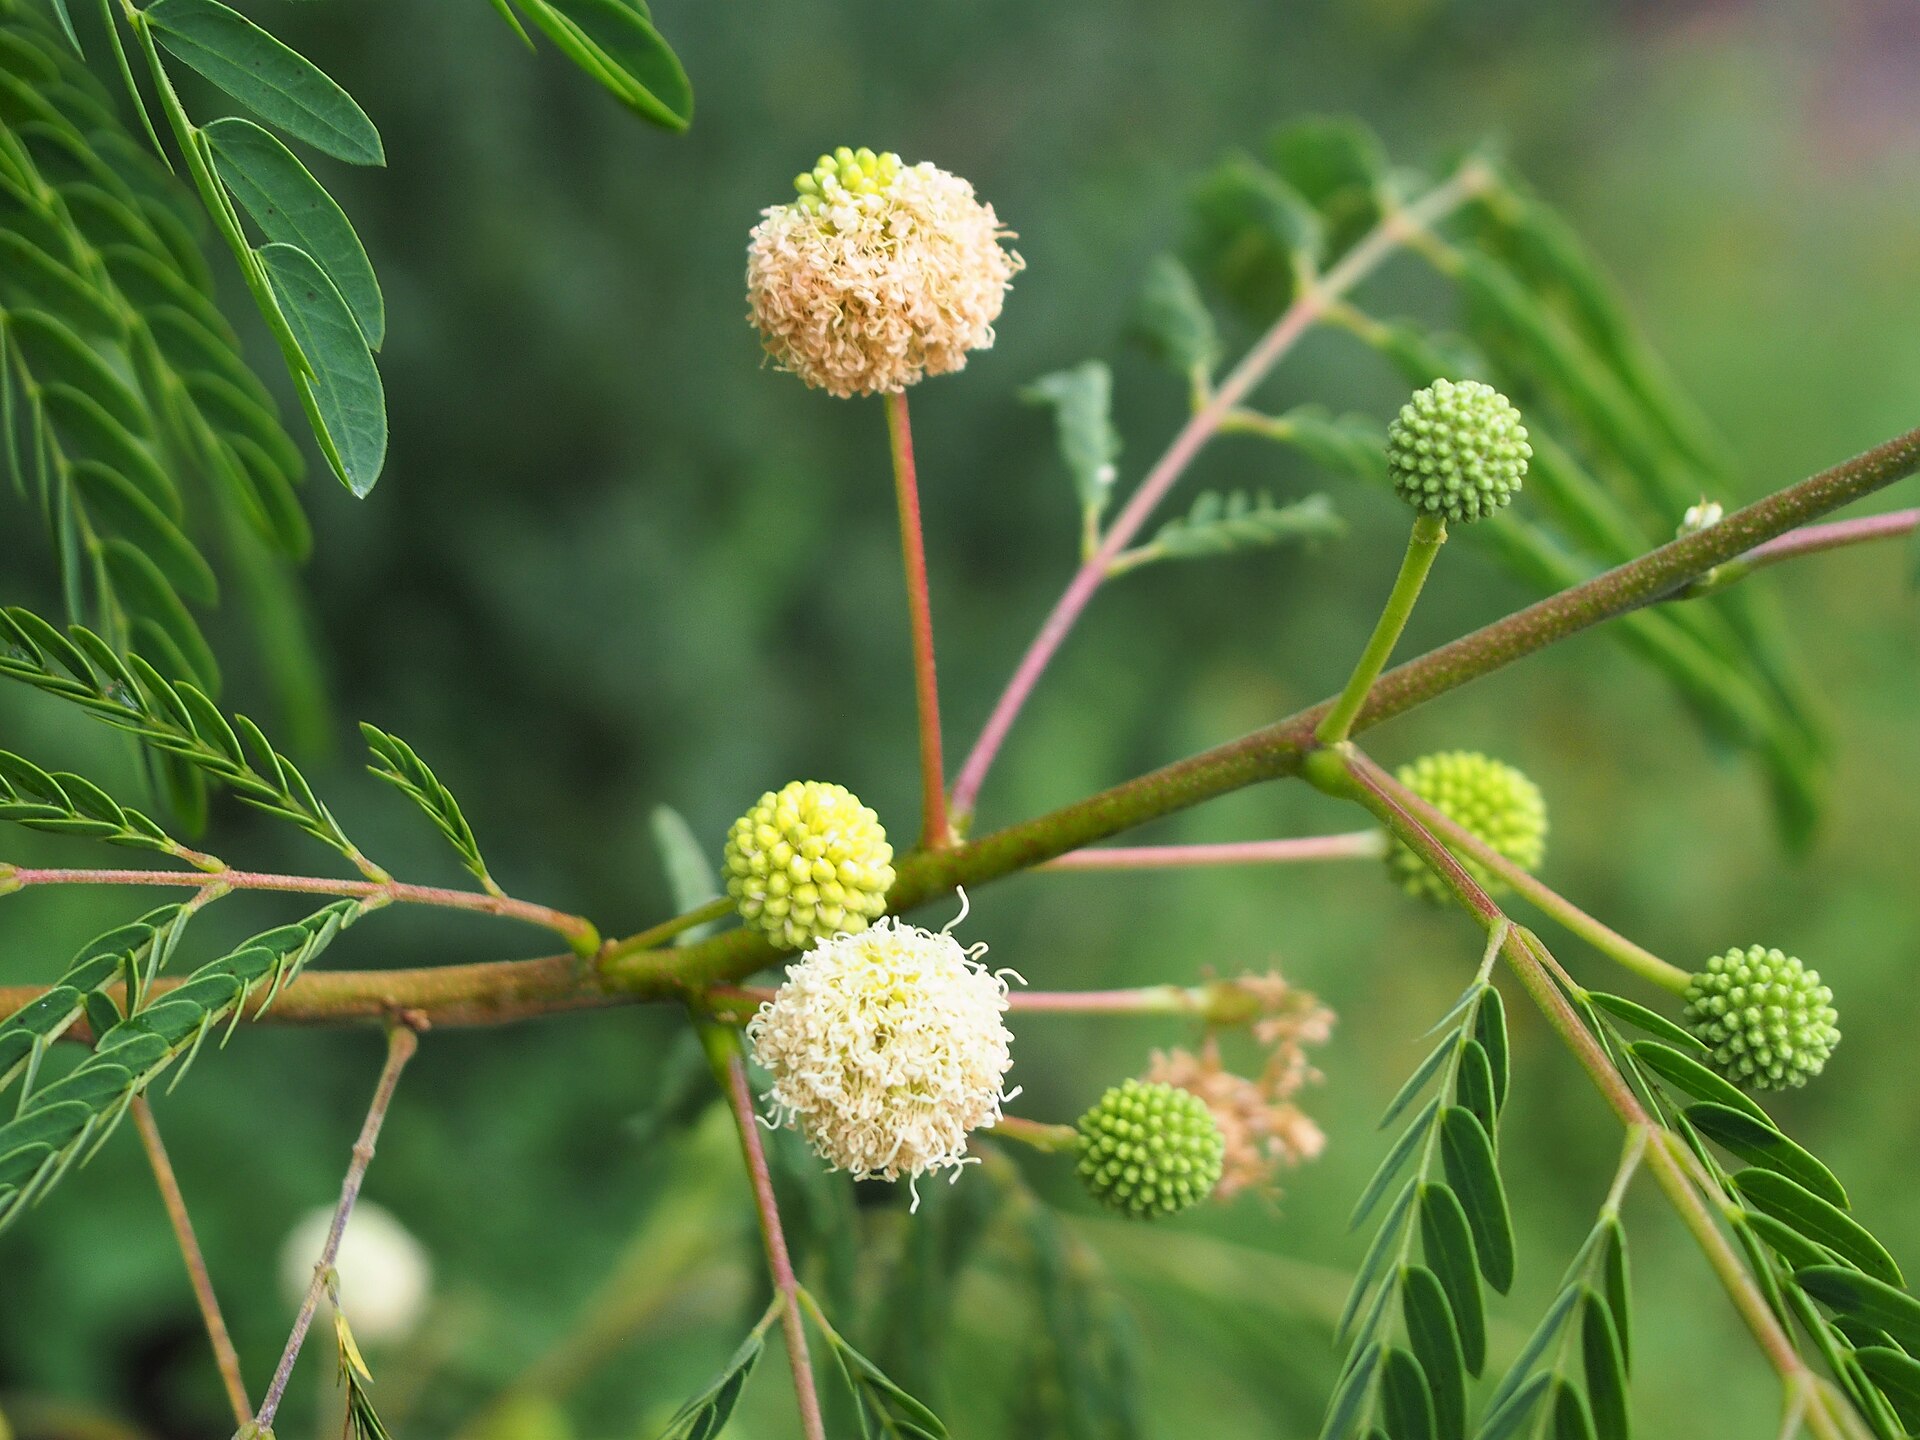
Leucaena lecocephala; photo by Agnieszka Kwiecien-Nova via WikiMedia

They report that the most widely distributed species is river tamarind, Leucaena leucocephala (Fabaceae); it occurs on all nine islands. Another seven species are found on seven of the islands: Casuarina equisetifolia (Casuarinaceae); Eichhornia crasssipes (Pontederiaceae); Megathyrsus maximus (Poaceae); Melaleuca quinquenervia (Myrtacea); Ricinus communis (Euphorbiaceae); Spathodea campanulata (Bignoniaceae), Terminalia catappa (Combretaceae).

The density of invasive plants per square kilometer varies considerably among the islands. The Virgin Islands (US and British) rank second highest at 0.245 / km2. Puerto Rico doesn’t stand out. As noted above, each island has a distinct invasive flora. The pair of islands which share the highest number of species (122) is Puerto Rico and the Virgin Islands (Rojas-Sandoval et al. 2017). I suggest it might be informative to explore whether these islands’ century-long ties to the United States influenced trade pathways and planting choices, thereby leading to this similarity.  

Rojas-Sandoval et al. (2017) report that 31% of the invasive plants (162 species) are herbs; 20% (102 species) are trees; 16% (80 species) are shrubs; 15% (77 species) are grasses; 13% (67 species) are vines; 3% (15 species) are succulents; 2.5% (13 species) are aquatics. Three-quarters are perennials. These plants occur primarily in human-altered habitats: 98% (506 species) in ruderal areas; 61% (314 species) in seminatural areas; 35% (138 species) in agricultural areas. Only 5% (27 species) are found in mature forests.

Nineteen of the species are listed among the “world’s worst alien invasive species”. For example, six of the eight most widely distributed species (above) are invasive in Florida also.

Seventy-five percent of the invasive plant species have escaped from cultivation. According to Rojas-Sandoval et al. (2017), half of these were introduced as ornamentals; another third were introduced for various agriculture and forestry purposes. Finally, 7% were deliberately planted in natural ecosystems for some purpose such as erosion control. They suggest that repeated introduction of some of these species – especially the ornamentals – might increase propagule pressure and thus their probability of establishing.

Generalities About Biology on Puerto Rico

Puerto Rico is the smallest island of the Greater Antilles at ~ 9100  km2 (5,325 mi² / 1,379,000 ha) (Rojas-Sandoval, Presley, and Willig 2026). It is 39% forest, 32% grassland, 13% woodland and shrubland, 11% urban, 3% herbaceous wetlands, 1% forested wetlands, 1% inland water, < 1% natural barrens (Castro, Quinones, and Gould 2016).

Puerto Rico is relatively poor in species richness compared to mainland tropical areas. In one example, a plot in a Puerto Rican wet forest had half the number of freestanding woody species as a comparably-sized area in central Panama. Puerto Rico lacks large herbivores and predators. Still, Puerto Rico is much more diverse than other more isolated islands, e.g., the Hawaiian Islands (Zimmerman, Rojas-Sandoval, and Shiels 2021). There are 2,780 species of plants and 361 native vertebrates, including 277 birds, 52 reptiles, 19 amphibians, and 13 mammals (Castro, Quinones, and Gould 2016).

This biodiversity reflects the island’s highly varied topography – elevations range from sea level to 1338 m – and rainfall. Areas in the south and southwest receive ~800 mm while the high-elevation areas in the northeast are drenched by more than 4000 mm.

Unlike in most tropical areas, forests on Puerto Rico are regrowing due to abandonment of agriculture. Forest cover has increased from less than 6% in the 1950s to more than 55% by 2014. These regenerating forests contain a mixture of native and non-native species in a mosaic of forest at various stages of succession (Rojas-Sandoval, Presley, and Willig 2026). Potter et al. (2022) reported that two-thirds of Puerto Rico’s forests comprised novel tree assemblages.

Invasive species

A decade ago, Puerto Rico had 176 invasive plant species – 32% of the island’s flora. They comprised 44 herbs, 35 grasses, 33 trees, 28 vines, 19 shrubs, and 5 succulents. In this category, Puerto Rico ranks higher than other islands in the Greater Antilles e.g. Jamaica (21%), Dominican Republic (18%), and Cuba (12%) (Rojas-Sandoval et al. 2017; Rojas-Sandoval and Acevedo-Rodríguez 2015).

Three studies have addressed invasive species on “la Isla del Encanto”. They differ in in geographic scope, data, and study objectives.

Zimmerman, Rojas-Sandoval, and Shiels (2021) addressed biological invaders in all taxonomic groups, not just vascular plants. However, their analysis was limited geographically to the Caribbean National Forest (CNF; popularly known as El Yunque). This study was based on published literature, museum and herbarium collections, local and academic experts’ experience, and personal field observations. They concluded that there were some worrisome trends but no strong evidence that the National Forest’s ecosystem was in danger of fundamental change as a result of invasive species. However, they admit data were limited and called for systematic surveys and detailed studies. This need is particularly acute because of the ecological importance of El Yunque, which is one of the few (and the most important) remnants of original native forest on Puerto Rico.

Potter et al. (2022) relied on data collected as part of the USFS Forest Inventory and Analysis (FIA) survey. The survey evaluates 341 permanent plots every 5 years. They assessed trees (no other kinds of plants) in forested areas across the island, not just in the CNF. They usually attribute invasive trees’ prevalence largely to the land-use history, i.e., reforestation of formerly agricultural lands. These scientists emphasize the importance of recent land-use history in determining where non-native tree species occur. They do not offer an overall assessment of the trajectory of invasions.

A more recent analysis by Rojas-Sandoval, Presley, and Willig (2026) was also island-wide and included all woody plants with dbh ≥ 2.5 cm, i.e., trees and shrubs. Noting that invasion intensity is steadily increasing in Puerto Rico’s forests, they concluded that the threat to Puerto Rico’s native biological diversity is greater than did the earlier studies.

Relying on the FIA surveys has the advantage of providing statistically valid data. However, this survey has two drawbacks as regards assessing plant invasions. First, the FIA inventory data don’t evaluate species in the understory, i.e., herbs, small shrubs, or vines. These species might also alter long-term successional trajectories (Rojas-Sandoval, Presley, and Willig (2026). Second, the FIA inventory is not designed to detect even woody plant species in the early stage of invasion, i.e., those that occur only as small seedlings on a few inventory plots (Potter et al. 2022). 

El Yunque

Invasive Plants

Zimmerman et al. (2021) report that 168 non-native plant species from 135 genera and 57 families are established in the National Forest  – at varying levels from “naturalized” to fully invasive. Of these, 77 species (~46%) had previously been listed as invasive on Puerto Rico. Twelve were hangers-on from crops planted in the past (e.g., coffee, mango, and breadfruit). They considered most of these non-invasive because they hadn’t increased strongly during a 10-year study. They named one possible exception, Simarouba amara, a timber tree, which had increased in numbers in areas of less intense land use after hurricanes in late 1990s. However, this species has not been mentioned as problematic by any other study.

El Yunque (CNF) is home to 37 of the non-indigenous plant species, including 14 vines, nine herbs, and eight grasses. These plants are described as colonizing primarily disturbed areas (e.g., landslides), wastelands, river edges, and roadsides.

The non-native species present in the regrowing forests vary by forest type – as would be expected given the large differences in rainfall. In the subtropical dry forest the principal invasive plants are river tamarind (Leucaena leucocephala) and Prosopis juliflora (Rojas-Sandoval, Presley, and Willig (2026). The former is one of the most widespread and common of the highly invasive non-native tree species throughout the Caribbean. On Puerto Rico, L. leucocephala is documented on 12.6% of 294 forested plots, 40% of plots in this biome. P. pallida (algarroba) is recorded on 10.9% of all survey plots, 27.1% of plots in the biome. Invasions in the dry forest are sometimes arrested by chronic disturbance – presumably fire (Potter et al. 2022). However, the authors do not report which species – native or introduced – come in after the disturbance.

The subtropical moist forest is presumably the biome most affected by previous agricultural efforts.  African tuliptree (Spathodea campanulata) occupies 41.8% of survey plots in this biome. Rose apple (Syzygium jambos) is found on 36.4% of these survey plots (Potter et al. 2022).

Invasive trees in the subtropical wet and rain forests biome included Erythrina poeppigiana and two species also found in the moist biome – Spathodea campanulate, and Syzygium jambos. S. campanulata is found on 33.9% of the plots in this biome (Potter et al. 2022). Zimmerman et al. (2021) call our attention to an herb, Selaginella willdenowii. They call this ornamental spikemoss one of most aggressive plant invaders in the CNF.

There is a difference of opinion on the threats posed by Spathodea campanulata. Potter et al. report that S. campanulata is found on 6.1% of all plots surveyed – half or less of plots invaded by the dryland species Leucaena leucocephala and Prosopis juliflora (and the S. campanulata plots are spread across two much larger biomes – moist and wet forests). S. campanulata is also shade intolerant so Potter et al. believe it might decline in the future as other species overtop it. The conflicting opinion is offered by Rojas-Sandoval, Presley, and Willig (2026). They call Spathodea campanulata a key driver of native biodiversity loss and homogenization in moist and wet forests. They note that the species has broad ecological tolerance and can proliferate after hurricanes. They found the species to already be significantly influencing native forest distinctiveness and composition – and to be increasing in abundance.

Potter et al. (2022) considered rose apple (Syzygium jambos) to pose a higher threat since it is shade tolerant and can form dense, monotypic stands under closed canopies – which S. campanulata cannot. Zimmerman, Rojas-Sandoval, and Shiels (2021) agree that where it occurs in areas of secondary forest near stream beds, S. jambos outcompetes other species. Rojas-Sandoval, Presley, and Willig (2026) note the species might potentially contribute to homogenizing biodiversity. A new development might counter this threat: the accidental introduction of guava/ohia rust (Austropuccinia psidii); it has been highly fatal to rose apple populations in Hawai`i.  Both Zimmerman et al. and Rojas et al. mention this possibility but I have not seen a more recent discussion of whether this is occurring.

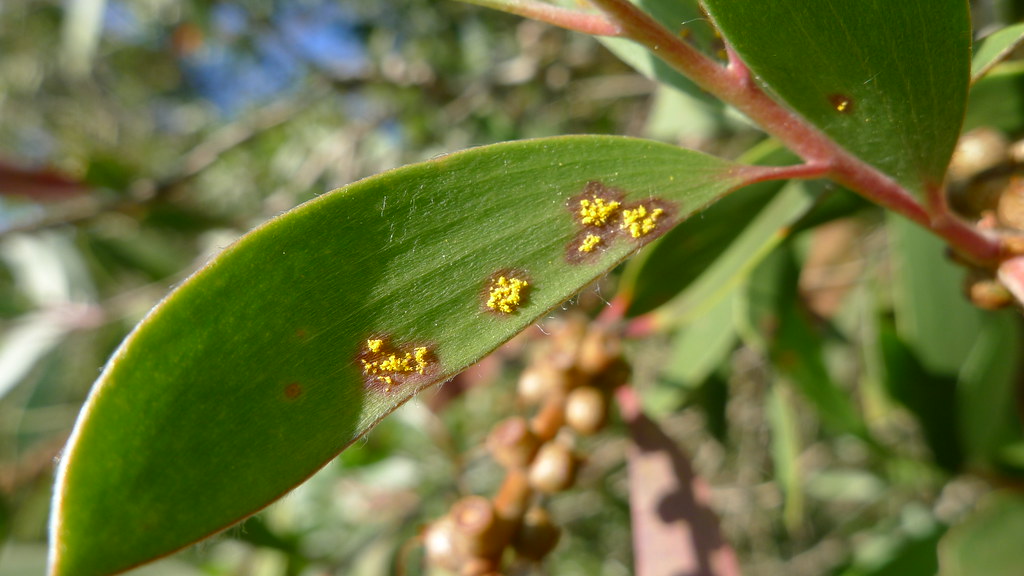
myrtle rust on Syzygium jambos; photo by Smallbiologie via Wikimedia

Zimmerman et al. (2021) say several invasive vines are established in El Yunque. The vines respond quickly to the disturbances caused by the region’s frequent hurricanes. Seven of the 14 species in the CNF are morning glories in the Ipomoea genus. Other locally abundant non-native vines are Epipremnum pinnatum, Pueraria phaseoloides, Dioscorea alata, Thunbergia alata, and Thunbergia fragrans.m

Potter et al. (2022) defined invasive tree species as those exhibiting 60 – 75% of stems in the “small” diameter categories (less than 12.5 cm dbh). Fifty-seven non-native tree species in old-growth and regenerating forests it this definition. They considered 17 of them as highly invasive, 16 as potentially highly invasive, and two as moderately invasive. That is, 35 of 57 nonnative tree species, or 60%, are actually or potentially bioinvaders. While on the continent only seven non-native tree species occurred on at least 2% of FIA plots across the ecoregions in which they were inventoried, on Puerto Rico 21 species (38%) occurred on at least 2% of the FIA plots. Potter et al. (2022) could not assess the invasiveness of eight additional species that occurred only as small stems on a couple of survey plots.

Potter et al. (2022) note the possibility of conflicting views about the invaders: some of the moderately to highly invasive species provide timber and non-timber forest products. These include S. campanulata, L. leucocephala, Syzgium jambos, and Mangifera indica (mango).

Rojas-Sandoval, Presley, and Willig (2026) also analyzed FIA data to assess how non-native tree species affect the biodiversity and composition in three forest types: dry, moist, and wet forests. Unlike Potter et al. (2022), they found that non-native tree species are reshaping native tree assemblages in Puerto Rican forests, leading to significant declines in native species abundance, richness, evenness, and diversity.

The transformation is greatest in the dry forest; there, native richness has declined by more than 90% by some measures. Native communities have become depauperate, dominated by a few species. In subtropical moist forest, native richness peaked at low to moderate invasion levels, then declined. S. campanulata is the dominant non-native species; as noted above, it is found on 41.8% of survey plots in this biome. In subtropical wet forests, native species richness and diversity were highest in uninvaded and lightly invaded plots, followed by marked declines at higher levels of invasion. This is largely driven by that one species, S. campanulata (found on a third of the survey plots in this biome).

The dry forest suffered the greatest proportional loss of biodiversity, including the largest proportional declines in native species richness. Wet forests also experienced strong declines in native richness & abundance. However, since wet forests had much higher initial diversity & structural complexity, their proportional decline in biodiversity is less. Thus, invasion effects differ among forest types depending on initial diversity, resource availability, land-use history, successional stage, and community composition.

Invasion can make individual plots diverge locally through loss of some rare species or gain of different non-native species. If this happens across the study site, the compositional heterogeneity at broader scales is simultaneously reduced. This results in landscape-level biotic homogenization.

Rojas-Sandoval, Presley, and Willig (2026) say homogenization effects are particularly concerning in insular ecosystems, where high endemism and ecological specialization make native biotas especially vulnerable to displacement.

To their surprise, the key driver on Puerto Rico is the increasing abundance of the non-native trees, rather than non-native species richness (Rojas-Sandoval, Presley, and Willig. 2026).

RECOMMENDATIONS

Potter et al. (2022) advise limited efforts to eradicate or control the eight species that occurred only as small stems on a couple of survey plots. These are probably incipient invasives. They name specifically Schinus terebinthifolius (Brazilian pepper) – a species already recognized as moderately invasive in Hawai`i and seriously invasive in peninsular Florida. In 2019 USDA APHIS approved release of two biocontrol insects in Florida targetting Brazilian pepper.

infestation of Brazilian pepper in the Florida Everglades; photo courtesy of Tony Pernas, National Park Service

I recommend that, in order to avoid having to consider importing those biocontrol agents to Puerto Rico, island conservation stakeholders should focus eradication efforts on this species now while it is still – apparently – not widespread.  

Rojas-Sandoval, Presley, and Willig (2026) are bolder. They call for implementation of more effective policies to prevent additional introductions and spread of the invasives already on Puerto Rico or nearby islands. They suggest that officials focus on the species named in their dataset. In addition, scientists should also collect data on understory dynamics to get a more comprehensive assessment of bioinvasion in the forest. Rojas-Sandoval et al. (2026) also urge implementation of policies aimed at reducing anthropogenic disturbances in these fragile ecosystems. One component of this program is for those responsible for forest management, conservation, and climate adaptation to incorporate invasion dynamics into their strategies. They remind us that Caribbean islands host extraordinary species richness – many of which are endemic. So protecting these biological riches is of global importance.

Preventing anthropogenic disturbance is likely to aid control of invasive plants. Zimmerman et al. (2021) found that the better-protected forests of the Caribbean National Forest was less invaded by vascular plants than were similar areas that had higher levels of human disturbance. However, this was not the case regarding invasive mammals and some invertebrates. Other than the passing reference to Austropuccinia psidii on Syzygium jambos, none of the studies considered pests or pathogens hosted by trees or other plants. 

Other Taxa

Zimmerman et al. (2021) also evaluated invasive animal species. They report that six species of vertebrates are invasive in Caribbean National Forest. Black rats (Rattus rattus), mongoose (Herpestes auropunctatus), and feral cats (Felis catus) are widespread through both disturbed and undisturbed mature forest. Each threatens many native species. The black rat also preys on seeds of several native tree species. House mouse (Mus musculus) is also very common, but restricted to roadside habitats. Cane toad (Rhinella marina) and green iguana (Iguana iguana) are also present. The green iguanas was introduced relatively recently and is rarely observed in CNF. Cane toads have been established much longer. Zimmerman et al. (2021) report no impacts.

Surprisingly, they report no introduced bird or fish species in El Yunque, even the species are common on the island and in parts of the Forest having a history of anthropogenic disturbance.

Two invertebrate bioinvaders are reported as ubiquitous in the National Forest: a hybrid honeybee and Aedes aegypti mosquito. The Africanized honeybee has evolved gentle behaviors and is no longer a great threat to cavity nesting birds, including the endangered Puerto Rico Parrot (Amazona vittata). Two species of introduced earthworms, Pontoscolex corethrurus and Ocnerodrilus occidentalis, are widespread in El Yunque; a third, Drawida barwelli, is found only in lower-elevation forest areas outside NF. The earthworms alter biogeochemical cycling in the soil, which might further influence plant community dynamics. Non-native slugs and snails do not appear to be spreading rapidly or damaging native plant species. Zimmerman, Rojas-Sandoval, and Shiels (2021) warn that additional invertebrates might be of concern in the future, since they can expand rapidly after forest destructions caused by hurricanes.

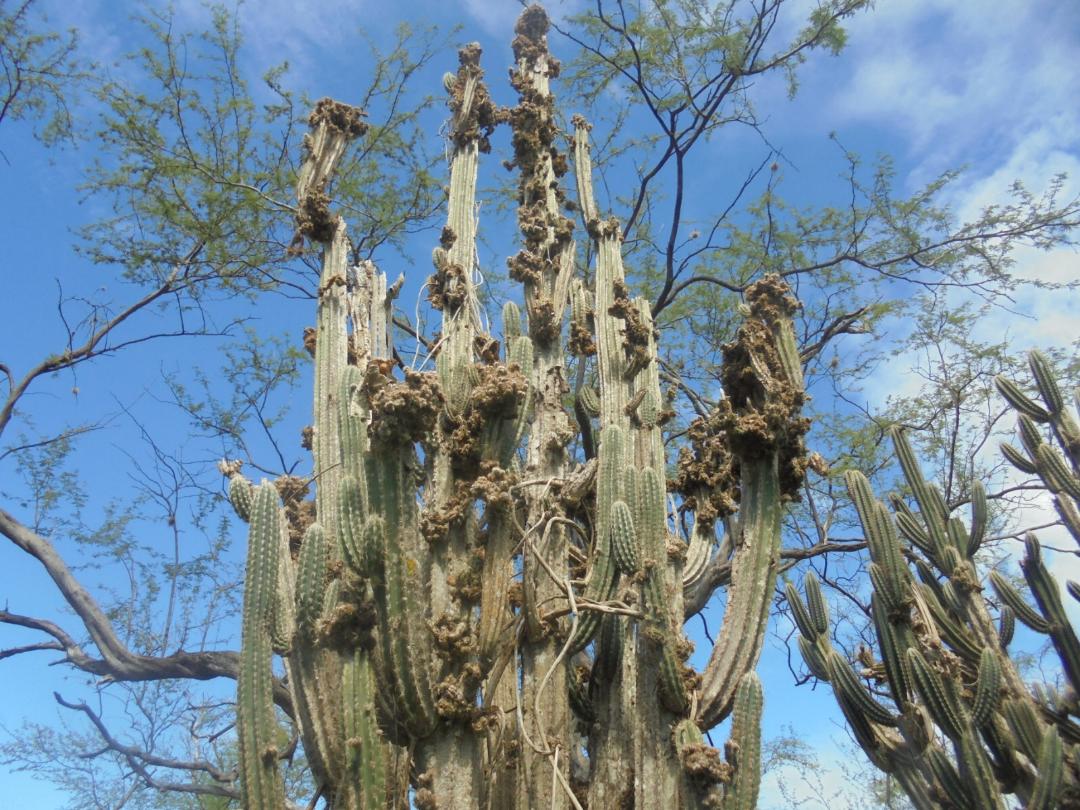
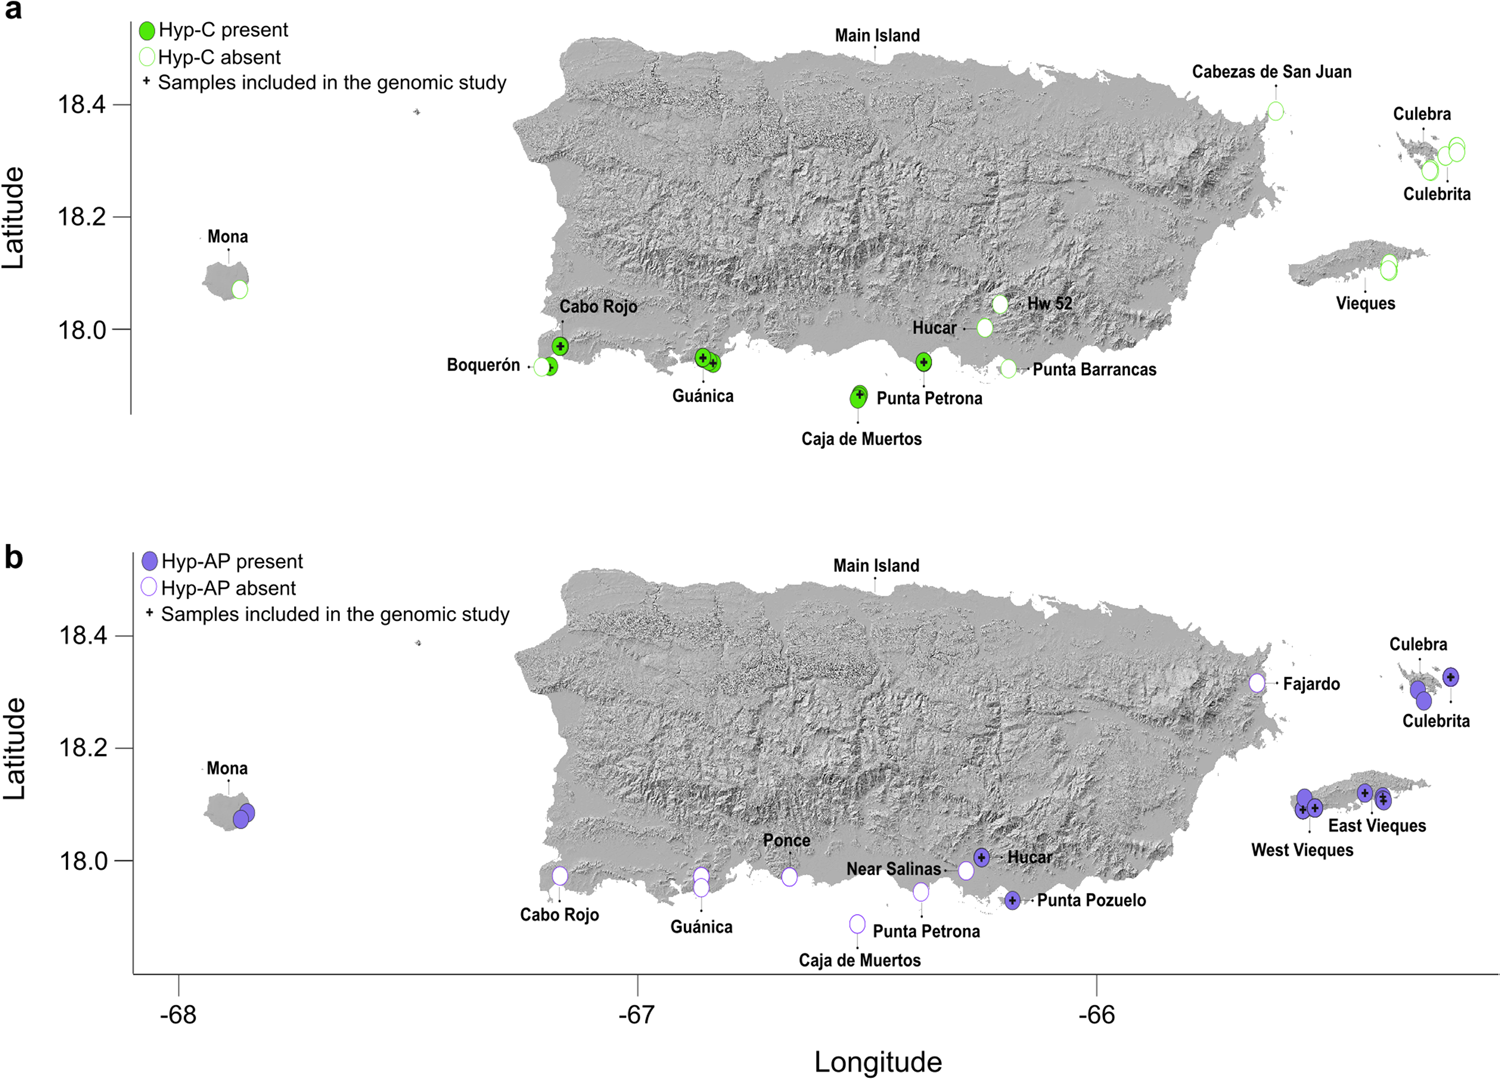
See also the brief summary of invasive species on Puerto Rico included in the Regional Summary Appendix for the Southeast in Poland et al. (2019). I note mentions of the South American Harrisia cactus mealybug (Hypogeococcus pungens, which is killing columnar cacti in the islands’ dry forests.  

SOURCES

Lugo, A.E., J.E. Smith, K.M. Potter, H. Marcano Vega, C.M. Kurtz. 2022. The Contribution of Non-native Tree Species to the Structure and Composition of Forests in the Conterminous United States in Comparison with Tropical Islands in the Pacific and Caribbean. USFS International Institute of Tropical Forestry General Technical Report IITF-54.

Poland, T.M., Patel-Weynand, T., Finch, D., Miniat, C. F., and Lopez, V. (Eds) (2019), Invasive Species in Forests and Grasslands of the United States: A Comprehensive Science Synthesis for the United States Forest Sector. Especially the Appendix on the Southeast and Caribbean. Springer Verlag. Available gratis at https://link.springer.com/book/10.1007/978-3-030-45367-1

Potter K.M., Riitters, K.H. and Guo. Q. 2022. Non-native tree regeneration indicates regional and national risks from current invasions. Frontiers in Forests and Global Change Front. For. Glob. Change 5:966407. doi: 10.3389/ffgc.2022.966407

Rojas-Sandoval, J., R.L. Tremblay, P. Acevedo-Rodriquez, H.D. Soltero. 2017. IAS plant species in the West Indies: geog, ecological and floristic insights. Ecology and Evolution 2017; 1-12

Rojas-Sandoval, J., Presley, S.J. and Willig, M.R. 2026. Increasing non‑native tree abundance reshapes biodiversity and composition of tropical forests. Biol Invasions 28, 84 (2026). https://doi.org/10.1007/s10530-026-03802-w

Zimmerman, J.K., J. Rojas-Sandoval, and A.B. Shiels. 2021. IAS in PR: The View From El Yunque. Front. Ecol. Evol. 9:640121. doi: 10.3389/fevo.2021.640121

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Protecting forests’ ecosystem values: minimize disturbance & curtail nearby planting of non-native species

old-growth forest in Tioresta Research Natural Area, Allegheny National Forest (Pennsylvania); photo by Nicholas T via Flickr

The implied or explicit recommendations are not new. But they are supported by new data!

Several measures of forest health drawn from survey plots of the Forest Inventory and Analysis (FIA) show that federally-owned forested lands – in both National forests and National parks – are healthier than neighboring forests under different ownership. Forest inventory plots in federal forests have significantly greater tree species and structural diversity and evenness; basal area and biomass per hectare; and seedling density. They are also less invaded by non-native plants. These findings hold across the continental United States, four regions (North, South, Rocky Mountains, and Pacific Coast) analyzed separately, and 22 common forest types.

The consistent finding of more “mature forest” features in eastern National parks and National forests – regardless of longer-term land-use histories (Potter et al. 2026b) – seems to me to indicate that recent and current management practices might overcome influences of centuries of pre-protection land use histories of exploitation and degradation.

1. Forest Health Inside vs. Outside Federal Forested Lands

Legally designated USFS National forests comprise ~19% of the Nation’s total forest area (~59 million out of 310 million hectares). Since adoption of the Forest and Rangeland Renewable Resources Act of 1974, the National Forest System (NFS) within USDA has been managed to maintain “appropriate forest cover . . . to secure the maximum benefits of multiple use sustained yield management in accordance with land management plans”. The Department of Interior’s National Park Service units are managed to conserve unimpaired the natural and cultural resources and values in the system for the enjoyment, education, and inspiration of this and future generations (National Park Service “Organic Act” of 1916).

Potter et al. 2026b assessed the ability of National forests to provide ecosystem services and forest products in the face of dramatically increasing threats:  (1) more intense and frequent wildfires; (2) uncharacteristically long and hot drought conditions; (3) mortality and compositional changes caused by invasive forest pests; (4) competition from invasive plant species; and (5) forest fragmentation and conversion to other land uses. To do this, they asked whether National forests (1) have greater biodiversity – as measured by species and structural diversity; (2) are denser and encompass more biomass; (3) experience more regeneration; and (4) are less invaded by non-native plants. The FIA surveys were carried out from ~2010 to ~2022. As noted, they analyzed each comparison across the conterminous states, the four regions, and the 22 forest types. 

Potter et al. (2026b) and an earlier study by Miller et al. (2016) agree that ownership determines forest management, specifically the level of anthropogenic disturbance allowed. Miller et al. demonstrated that, in the eastern United States, forests in National parks have greater live tree basal area, a larger volume of coarse woody debris, and greater proportions of late-successional tree species than nearby forests. They also have lower rates of tree growth and mortality.

Potter et al. (2026b) found that all biodiversity indicators except number of saplings per hectare were higher for plots inside the NFS than neighboring forests under other ownerships. This was true across the continent and in all four regions.

In some of the 22 forest types the indicators were particularly strong. Thus, basal area was notably higher on NFS forests populated by loblolly/shortleaf pine, Western larch, hemlock/Sitka spruce, maple/beech/birch, and oak/hickory forest types. Tree species richness was significantly higher on NFS plots for Western larch, elm/ash/cottonwood, longleaf/slash pine, pinyon/juniper, and loblolly/shortleaf pine. Differences in regeneration were seen most prominently in loblolly/shortleaf pine, oak/hickory, oak/pine, and white/red/jack pine. The authors do not speculate on the reasons.

a large loblolly pine in Congaree National Park; via Picaryl

The FIA data showed that invasive plant richness and cover were both greater on plots outside National forests across the Continent and in all four regions. However, invasive plant richness did not differ by ownership for some specific forest types: elm/ash/cottonwood, pinyon/juniper, Western larch, and hardwood woodlands. (National parks are even less invaded by non-native plants than National forests; see below.)

2. Regions Differ – Why?

Geographic regions differed noticeably. Tree species richness and evenness; diversity and evenness of tree height classes; biomass/ha; seedlings and saplings per hectare; and invasive plant diversity and cover were higher in the East – in both USFS Northern and Southern regions. Tree species richness was by far highest in the South – especially in the southern Appalachians and on the Cumberland Plateau. Seedling density was highest in the North, moderately high in the South. In the North, tree species and tree height evenness were both higher on non-federal lands.

Invasive plant richness was highest in some parts of the South. [See a more detailed discussion of invasive plants below.] Tree diameter class diversity and evenness were significantly higher in the West. Basal area was by far the highest in the northern part of the Pacific coast region (Washington, Oregon, and California.). Seedling density was moderately high in some National forests in the Rocky Mountains. Tree diameter evenness was higher outside National forests in the Rocky Mountains.

These differences had been expected given the marked regional dissimilarities in floristic, climatic, and edaphic factors, as well as ownership patterns.

Potter et al. (2026b) report that tree recruitment was stronger in the East than the Rocky Mountain and Pacific coast regions. I wish they had discussed how this finding relates to earlier findings (Potter and Riitters 2022) that numbers of species experiencing poor regeneration were highest in the Southeast, followed by the Northeast and Midwest. Miller et al. (2023) also found that tree regeneration was poor in National parks from Virginia to Maine. The latter study attributed this failure to a combination of browsing by overabundant deer and competition by invasive plants. The latter is presumably even more important in national forests, which are invaded by non-native plants at twice the rate of national parks. Nonfederal forests are invaded at even higher rates – up to 3 times greater. [See here for a study of improve regeneration in National parks which control their deer populations.]

Potter et al. (2026b) note that the higher forest health indicator values for NFS forests prevailed across the Continent despite notable differences in land-use and management histories and landscape contexts. Most NFS land in the West was put under federal management before arrival of European pioneers, so more of their groves are classified as old-growth or mature. In the East, nearly all lands incorporated into the National Forest System were privately owned until they were purchased in the 20th Century. At that time these forests were often highly degraded. Not only did the eastern National forests have to recover from overexploitation; they are still typically embedded in a matrix of other land ownerships, often largely cleared of trees.

In their analysis, Potter et al. (2026b) controlled for differences in site productivity and some environmental conditions e.g., elevation and slope, but not soil or hydrological conditions. So they believe that the suite of environmental factors do not explain the “older” attributes of eastern forests managed by the USDA Forest Service and USDI National Park Service,. These attributes generally include a more complex forest structure; higher tree species richness; and greater basal area and density of live trees (Miller et al. 2016). 

What differs is management. Miller et al. (2016) say explicitly that protection from forest harvesting for many decades probably is an important explanation of why forests in the eastern National parks have greater tree species diversity than forests owned by other parties. Potter et al. (2026b) instead emphasize the impacts of different land-use histories outside of National forest boundaries. Much of this land (especially in the East) has experienced continuous, centuries-long agriculture and residential development and more acute disturbance pressures associated with higher human population density. They also note that managers of non-federal forests goals often call for harvests or other active management – which can reduce forest structure, species richness, size of live trees, presence of downed woody debris, etc.    

I note that the consistent finding of more “mature forest” features in eastern National parks and National forests – regardless of longer-term land-use histories (Potter et al. 2026b) – indicates that recent and current management practices might overcome older influences. Many of these forests have enjoyed protective management for less than a century; the Forest and Rangeland Renewable Resources Act of 1974 was adopted just 50 years ago. I assert that the decisive factor might be the much lower presence – although not absence! – of deliberately planted non-native plant species on federal properties. [Again, see a more detailed discussion of invasive plant issues below.]

Potter et al. (2026b) also comment that regeneration on NFS land is almost exclusively natural. As discussed above, they consider this regeneration to be successful, in that seedlings generally are being produced in greater numbers than on surrounding forests in other ownerships. Again, I would like to learn how this finding relates to the earlier study by Potter and Riitters (2022).

Potter et al. (2026b) state that National forests benefit from their greater size and stability of management goals. These are necessary for large-scale approach to conserve or imitate the processes that create diversity

As Potter et al. (2026b) note, in the East, reserved areas like National forests (or to a greater extent, National parks) represent a small proportion of the landscape. Their distinctness from neighboring forestlands emphasizes their ecological value.  They call for managers to be alert to potential invasions of non-native plants or tree-killing pests from the surrounding agricultural and developed land. In the West, private forests abut federal forested lands less often and thus have less influence on the status of forest health indicators on National forests.

3. Plant Invasions in Forests

Several studies by Kevin Potter, Kurt H. Riitters and colleagues have documented the extent of plant invasions in America’s forests.  Data supporting these studies come from the same forest plot surveys conducted under the Forest Inventory and Analysis (FIA) program.

The region most invaded is Hawai`i: 83% of FIA plots have one or more invasive plant species. The region that ranks second is the East, specifically the 37 states comprising the USDA Forest Service’s former Northern and Southern regions. Nearly 53% of FIA plots in this region have one or more invasive plant species (Potter et al. 2024). FIA plots in the Rocky Mountain West had only 11% (Potter et al. 2026a).

student volunteers in Camp S.E.E.D. (Students Encouraging Environmental Recovery) program pulling invasive plants in Shenandoah National Park; via Picaryl

As noted above, invasive plants are particularly problematic in the South. There, invasive plants have been documented on 55.3 million hectares. In the Northern Region, an incomplete survey found invasive plants on 36.9 million ha. In some counties of the 37 states, 80% of inventoried forest plots contain invasive plants. Spread of these invaders is largely unchecked. The invasions’ extent and intensity are so great that their complete removal – or elimination of their impacts – is “practically impossible” (Potter et al., 2024; Potter et al. 2026a).

Plant invasions in eastern forests are undoubtedly worse than these data indicate because the records include only some of the non-native plant species present — those considered to be the worst invaders at the time regional lists were compiled (Potter et al. 2026a). Not included on the survey list are wavy-leaf basketgrass (Oplismenus undulatifolius), fig buttercup (Ficaria verna), shrub and creeping Euonymus, callery pear (Pyrus calleryana). Only one privet (Ligustrum vulgare) is included.

Furthermore, Bradley, Early and Sorte (2015) report that while non-native plant species are already more widely distributed than native species, the average invasive plant species inhabits only about 50% of its expected range.

Sites Most Heavily Invaded

Analyses of the FIA data reveal several overlapping definitions of which locations and situations have been invaded most severely. These factors are separate from the issue of ownership discussed above. Invasive plants are more numerous, widespread, and diverse in more disturbed or fragmented sites. One study found that 65% of plots that experienced greater fragmentation were invaded compared to 46% of plots that experienced low fragmentation. Invasion rates are highest in the “wildland-urban interface” (WUI). Unfortunately, the WUI is growing faster than any other land use type in the country – especially in the East (Potter et al. 2024). Because the East is so heavily developed, a plot’s distance from a road was nearly irrelevant. Furthermore, development in the WUI also promotes planting of non-native species that might then invade the nearby forest. See my more detailed discussion of these issues here.

Highly productive sites [defined as a site’s ability to grow industrial timber; Potter et al. 2026b] are also prone to invasion: 76% of highly productive plots were invaded compared to 40% of low-productivity plots. It is not known whether highly productive sites are inherently more invasible, or, instead, that such plots were converted to agriculture earlier, so exposed to human disturbance longer (Riitters et al. 2017).

A third analysis found that the best predictor of the odds that a site would be invaded was the site’s ecological province as defined by Robert G. Bailey in 1995 (Riitters et al. 2017)

Propagule Pressure: the Role of Deliberate Planting

Over 25 years (Reichard and White 2001) numerous scientists have documented the role of deliberate planting – especially ornamental horticulture – in facilitating introduction and spread of invasive plants. Kinlock et al. (2025) found that more than 1,600 plant species sold by nursery and seed catalogs over 200 years had “naturalized” somewhere in the continental 48 states. Fertakos and Bradley (2024) found that species were likely to establish if they were introduced to as few as eight locations. Beaury et al. (2023) found that half of 89 plant species recognized as invasive are sold in the same locations where they are invasive. Another 25 species are sold in an area that is currently unsuitable for those species, but that will become more suitable for invasion as temperatures warm.

Japanese barberry – invasive that is widely sold; photo by Matthew Beziat via Flickr

Both Potter et al (2024) and Potter et al. (2026a) note that the flora of suburban and rural residential landscapes is dominated by non-native plant species. I add that the people who live there promote plant invasions in various ways, including planting shrubs or flowers in the woods and dumping yard waste there. The older the human settlement, the more years for these plants to spread – assisted by birds, wind, or water. Go here for a more detailed discussion of these issues.

What Should We Do to Curtail Introduction and Spread of Invasive Plants?

a. Regulations The ornamental plant market – whether brick and mortar stores or internet sales — is interstate in scope. Regulations need to match (Beaury et al. 2023). This requires Congress to adopt a new federal law. Under the Constitution, the appropriate entity for regulating interstate commerce is the federal government. But the current statute (the Federal Noxious Weed Act) does not address long-established, widespread species.

States currently have the lead in regulating sales of horticultural plants. Beaury et al. (2023) and Evans et al. (2024) criticize state restrictions as outdated, limited to a few weeds that plague agriculture, and irregularly enforced. The result is a checkerboard of places where a species is offered for legal sale next to places where that sale is prohibited. Finally, the regulations are reactive; they rarely include plants in anticipation of their spread to new areas. Evans et al. (2024) urge state regulators to prioritize those species in the ornamental trade that are projected to remain or become abundant under evolving climate conditions.

b. Voluntary Actions

Potter et al. (2024) call for efforts to encourage homeowners to plant more native and environmentally friendly private landscapes. They concede the complication that some non-native – even invasive – species provide valued ecosystem and cultural services. They also suggest that local governments adopt land-use planning rules that protect forests of high conservation value. They do not discuss the extreme improbability of the latter action given the magnitude of predicted land-use changes in the country, powerful demographic factors driving them, and lobbying clout of affected economic interests, including the nursery industry.

Many citizen associations – native plant societies, regional or state invasive plant councils, etc. – are pursuing the education approach. (See the websites for state native plant societies, Southeast Exotic Pest Plant Council, Mid-Atlantic Invasive Plant Council, Midwest Invasive Plant Network, and Virginia Invasive Plant Coalition.) These voluntary efforts have yielded some success. But they have not resulted in adequate protection for our ecosystems.

c. Land-Managing Agencies

Many land-managing agencies work with local and regional groups to monitor and remove invasive plants, e.g., Blue Ridge PRISM. Databases that verify and post their findings, e.g., iNaturalist and EDDmapS can provide early warning of new invaders. See here for a discussion of these matters.

Blue Ridge PRISM removing English ivy; photo courtesy of Rowena Zimmerman, Director of Virginia Invasive Plant Coalition & Blue Ridge PRISM

Potter et al. (2026a) also suggest that the USDA Forest Service update the lists of invasive plants to be included in future FIA surveys. I agree. See above for examples of highly invasive species not now included.

Of course, the influence of plants on ecosystems is broader than invasive species. Dr. Douglas Tallamy has demonstrated that even non-invasive, non-native plants can disrupt food webs.

 SOURCES

Beaury, E.M., J.M. Allen, A.E. Evans, M.E. Fertakos, W.G. Pfadenhauer, B.A. Bradley. 2023. Horticulture could facilitate invasive plant range infilling and range expansion with climate change. BioScience 2023 0 1-8 https://doi.org/10.1093/biosci/biad069

Bradley, B.A., R. Early and C. J. B. Sorte. 2015. Space to invade? Comparative range infilling and potential range of invasive and native plants. Global Ecology and Biogeography

Evans, A.E., C.S. Jarnevich, E.M. Beaury, P.S. Engelstad, N.B. Teich, J.M. LaRoe, B.A. Bradley. 2024. Shifting hotspots: Climate change projected to drive contractions and expansions of invasive plant abundance habitats. Diversity and Distributions 2024;30:4154

Fertakos, M.E. and B.A. Bradley. 2024. Propagule pressure from historic U.S. plant sales explains establishment but not invasion. Ecology Letters 2024;27:e14494  doi: 10.1111/ele.14494

Kinlock, N.L., D.W. Adams, W. Dawson, F. Essl, J. Kartesz, H. Kreft, M. Nishino, Jan Pergl, P. Pyšek, P. Weigelt and M. van Kleunen. 2025. Naturalization of ornamental plants in the United States depends on cultivation and historical land cover context. Ecography 2025: e07748 doi:10.1002/ecog.07748

Miller, K. M., F. W. Dieffenbach, J. P. Campbell, W. B. Cass, J. A. Comiskey, E. R. Matthews, B. J. McGill, B. R. Mitchell, S. J. Perles, S. Sanders, J. P. Schmit, S. Smith, and A. S. Weed. 2016. National parks in the eastern United States harbor important older forest structure compared with matrix forests. Ecosphere 7(7):e01404. 10.1002/ecs2.1404

Miller, K.M., S.J. Perles, J.P. Schmit, E.R. Matthews, M.R. Marshall. 2023. Overabundant deer and invasive plants drive widespread regeneration debt in eastern United States national parks. Ecological Applications. 2023;33:e2837. https://onlinelibrary.wiley.com/r/eap

Potter, K.M and Riitters, K. 2022. A National Multi-Scale Assessment of Regeneration Deficit as an Indicator of Potential Risk of Forest Genetic Variation Loss. Forests 2022, 13, 19. https://doi.org/10.3390/f13010019.

Potter, K.M., K.H. Riitters, B.V. Iannone III, Q. Guo and S. Fei. 2024. Forest plant invasions in the eastern United States: evidence of invasion debt in the wildland‑urban interface. Landsc Ecol (2024) 39:207 https://doi.org/10.1007/s10980-024-01985-y

Potter, K.M., B.V. Iannone III, K.H. Riitters, Q. Guo, K. Pandit, C.M. Oswalt. 2026a. US Forests are Increasingly Invaded by Problematic Non-Native Plants. Forest Ecology and Management 599 (2026) 123281

Potter, K.M., Q. Guo, F.H. Koch, S. Lim-Hing, E.R. Matthews, and K. Pandit. 2026b. U.S. National Forests Are More Diverse, Denser and Less Invaded than Neighboring Forests. Forests 2026 17

Reichard, S.H. and P. White. 2001. Horticulture as a Pathway of Invasive Plant Introductions in the United States. BioScience 103. Vol. 51 No. 2. February 2021.

Riitters, K., K. Potter, B.V. Iannone III, C. Oswalt, S. Fei, Q. Guo. 2017. Landscape correlates of forest plant invasions: A high-resolution analysis across the eastern United States. Diversity and Distributions. DOI: 10.1111/ddi.12680

Tallamy, D.W. and K.J. Shropshire. 2009. Ranking Lepidopteran Use of Native Versus Introduced Plants

Conservation Biology, Volume 23, No. 4, 941–947 2009 Society for Conservation Biology

DOI: 10.1111/j.1523-1739.2009.01202.x

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Invasive species on the African Continent

We are beginning to get more information about invasive species on the African continent.

a flyer naming principal invasive ornamental plants in Kruger National Park

In several countries, the focus has been on threats to agriculture. Previous blog about horizon-scanning in Ghana. In Zimbabwe, N. Mudada and colleagues (2026; full citation and the end of this blog) found alarming, if not surprising, levels of risk to food production from introduced invasive plants. They investigated 1,668 human-aided transboundary plant introductions at 14 ports of entry and non-official crossing points over the course of four years.

They estimate that the 20,000 trucks that transported maize into the country over the four years carried over 20,700 metric tons of weed seeds and rubbish! They recorded detections of 11 species in eight orders. The pathways are familiar. As noted, several weeds were contaminants of grain shipments; Convolvulus arvensis in wheat for human consumption, Helianthus annus and Datura stramonium in maize for animal feed. Adenium obesum and Vitex agnus-castus were being smuggled for planting as flowers and ornamentals. (Vitex agnus-castus was also smuggled in passenger baggage for its medicinal properties). Several Lemna species (an aquatic plant) were also smuggled for planting as animal feeds.

In some cases, the focus is the threat to native ecosystems. I posted a blog the about threat of an introduced pathogen to trees in the remnant rain forests of Madagascar.

South Africa still has the lead in addressing invasive species. Regarding invasive plants specifically, the country has the benefit of more than 150 years of botanizing. The richness of the region’s flora is globally recognized. South Africa also has a long history of studying and managing invasive species, especially plants.

South African scientists and colleagues in Botswana, Eswatini, Lesotho, and Namibia have published four editions of the Flora of the Southern Africa region since 1984. In 2006, the PRECIS database of the South African National Biological Diversity Institute (SANBI) was combined with the Tropical African Plant Checklist published by the Conservatory and Botanical Garden of Geneva to create the African Plant Checklist and Database Project. It is continually updated. This is the first continental flora checklist for Africa; it fulfils countries’ obligations under the Convention on Biological Diversity’s Global Strategy for Plant Conservation.

For South Africa specifically, scientists have produced a national plant checklist that is updated annually.

The 2025 Checklist reports that 21,539 plant species are extant outside cultivation in the country; these comprise 20,204 indigenous species and 1,329 naturalized species. Thus, 6% of the total flora is non-indigenous. Of these, 649 (48.8% of the non-indigenous species, 3% of all plants) of them are invasive.

[Naturalized species are defined as species whose documented natural range does not include South Africa, but have overcome a biogeographic barrier and now sustain self-replacing populations for two or more life cycles or over a given period of time in the country. These populations are maintained without direct intervention by people, or despite human intervention. Invasive species meet the above definition plus produce reproductive offspring, often in large #s at considerable distances from the parent and/or site of introduction, and have the potential to spread over long distances.]

Since the previous checklist was published in 2006, botanists have identified 1,048 additional species – a 4.9% increase. Eighty-two percent of the newly identified species (865 species) are “naturalized”. Specifically, 414 new species are categorized as naturalized (a 31.1% increase), and 451 new species are classified as invasive (a whopping 69.5% increase). Le Roux and Klopper attribute these steep increases to active botanizing by SANBI’s Invasive Species Programme (begun in 2008), and the Southern African Plant Invaders Atlas Project (begun in 2010).

Of the 384 plant families present in South Africa, 350 contain at least some indigenous species. Thirty-four families contain only naturalized species. Among the 2,189 plant genera present, 459 (21%) contain only species that are non-indigenous.

Three families stand out because of the particularly high numbers of naturalized species: Fabaceae (143 species; 11% of all naturalized species), Asteraceae (140 species; 10%), Poaceae (123 species; 9%). Two of these families — Asteraceae and Fabaceae — are also the largest families among native South African plants. The third, grasses (Poaceae), ranks seventh in the list of most specious families indigenous to South Africa. The next group of families with high numbers of naturalized species has less than half as many invasive species: Myrtacae (55), Amaranthacea (52), Solanaceae (48). None of these families ranked within the top 20 families of indigenous plant species.

The genera with the most naturalized species were Solanum, Euphorbia and Acacia (all 24 or 23 species).

Acacia cyclops; photo by David M. Richardson

South African scientists are also exploring how to balance conflicting goals and perspectives when an invasive plant species has economic or social value. The example chosen by Mbobo et al. (2025) is guava (Psidium guajava) – a nutritious and popular tropical fruit grown commercially in South Africa, but also invasive along roadsides, watercourses and forest margins. Invasions are especially common in eastern parts of country; large monocultures are found in KwaZulu-Natal. Outbreaks have also been detected at five sites in Western Cape in riparian zones and at a hot spring. Mbobo et al. (2025) note that the microclimatic conditions at this last location differ from the broader conditions in the region – which are what most models would measure.

The scientists used models to predict where guava might invade – especially in large monocultures – and compared those areas to where the tree can be grown in cultivation with human inputs, e.g., irrigation. They then assessed whether six regulatory approaches would avoid restricting guava farming in areas at minimal or low risk while still protecting vulnerable locations. They also considered the amount of information required to implement the approach and costs of acquiring the information; and level of likely public acceptance. Mbobo et al. (2025) laid out the trade-offs between continuing to regulate planting of the species at the provincial level vs. at the municipal level. Prohibiting planting of guava in provinces where it is recorded as invasive allows some plantings near natural forests and riparian areas that are highly susceptible to guava invasions. On the other hand, nearly half of the prohibited area is outside the known or likely at-risk area. The provinces do allow exceptions through a permit process. Adopting more geographically limited rules by regulating at the municipal level would enable a tighter link to geographic areas at highest risk. However, this approach does not address long-distance seed dispersal by animals. Furthermore, the very detailed regulations might confuse stakeholders and complicate enforcement. Also, the models lack sufficiently fine spatial resolutions to predict invasible areas so accurately. Finally, the reduction in regulated area is minimal (~ 14%), so the economic benefits are unlikely to outweigh the significantly higher administrative costs and risk of allowing guava invasions in new sites.

Guava fruit on tree; Roenashy via Wikimedia

Gildenhuys et al. (2026) analyzed the factors that drive which non-native plants establish where. They assessed the roles of temperature, precipitation, urbanization intensity, urban area, travel time, year of city’s establishment, and human population density in determining which plant species are present in 54 urban centers in Western Cape Province. The cities have significant differences in climate: Mediterranean in the far southwest, warm temperate in the southeast, and semi-arid towards the interior. The expectation was that these drivers and assembly processes are influential at more advanced invasion stages when the species have already overcome some barriers to dispersal, so are now found in reasonably suitable habitats.

Gildenhuys et al. (2026) found temperature and precipitation were most important in determining plant species’ presence. This was especially true at the boundary between arid and mesic climates. These strong environmental gradients are the same ones which have driven high differences in native species presence across the province. [See pamphlet describing invasive plants in Cape Town.] This finding supports the “Goldilocks hypothesis”: that non-native plant species assemblages are driven by the same abiotic variables as native species assemblages. While did not directly study the “Biome decides hypothesis” (the composition of non-native flora is mediated by the biotic effects of native flora and fauna), Gildenhuys et al. (2026) doubt its applicability here because native species’ presence has probably been greatly reduced by the effects of urbanization.

Urbanisation intensity itself ranked third as a factor. Its effect was strongest at low to medium urbanization intensities. Because urbanization creates novel habitats, such as, “hardscapes” of paved surfaces that resemble deserts, their non-native plant assemblages are dominated by similar, urban specialist, species. At lower urbanization intensities a greater variety of habitats is available. Gildenhuys et al. (2026) conclude that urbanization acts primarily as a driver of opportunistic habitats for species at later invasion stages rather than as a filter of species introduction.

An earlier study found a similar effect from road density (often associated w/ urbanization) as an explanation for where specific woody non-native species establish. They do concede that larger urban areas might experience greater propagule pressure.

Gildenhuys et al. (2026) note that recent globalization of the plant trade has probably changed the specis planted in urban centers. For example, cities in the Western Cape are increasingly replacing English oak (Quercus robur) with more disease-resistant oaks. The change might reflect greater environmental awareness and regulations issued under the National Environmental Management: Biodiversity Act 10 of 2004. In newly established urban centers, fewer invasive species are being planted — at least among trees.

SOURCES

Gildenhuys, C.P., L.J. Potgieter, C. Hui, D.M. Richardson. 2026. Drivers of compositional turnover of the NIS urban flora in the W Cape, South Africa. Urban Ecosystems (2026) 29:51 https://doi.org/10.1007/s11252-026-01919-3

Le Roux, M.M., R.R. Klopper. 2025. Taking stock of South Africa’s flora. South African Journal of Botany 184 (2025) 571-579

Mbobo, T., D.M. Richardson, A. Datta, K.T. Faulkner, J.R.U. 2025. Wilson. Spatially-Differentiated Reg of NIS Can Be Improved Using Spp Distribution Models: Psidium guajava in South Africa as a Case Study. Diversity and Distributions. 2025 31:e70102 https://doi.org/10.1111/ddi.70102

Mudada, N., J. Chitamba, E. Nyangani, C. Chapano, N. Mapope,and W. Ngezimana. 2026. Weeds associated with cross border traffic, their approach and infestation rates in Zimbabwe.  ISABB Journal of Food and Agricultural Sciences. Vol. 12(1) January-June 2026. DOI: 10.5897/ISABB-JFAS2025.0192

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Factoids from recent publications

Agrilus auroguttatus

Agrilus genus

Hernández‐Gutiérrez, Nichols, and Kelly (2026) (full citation at the end of the blog) analyzed interactions between this genus of beetles and oaks (Quercus species). In this context, they report that 32 Agrilus species from Africa, Asia, Europe, and North and South America use 51 Quercus species as hosts in their native range. Eighteen (56.25%) use only Quercus hosts.

Oaks that host Agrilus species cluster in several clades, i.e., the entire Section Cerris and one clade of Section Ilex and two clades of section Lobatae. Clades where Agrilus hosts are underrepresented are Sections Cyclobalanopsis and Quercus &, surprisingly, two clades in Section Lobatae.  

Their analysis indicated that beetle-oak interactions involving all the 32 Agrilus species and 105 Quercus species in their study had a significant likelihood of being damaging. For example, northern red oak (Q. rubra) is already known to host six Agrilus species. Hernández‐Gutiérrez, Nichols, and Kelly (2026)’s analysis indicated that this tree species might be utilized by all 32 Agrilus species assessed. The tree’s wide distribution (both native and introduced) places it close to other known or probable hosts, which exacerbates the risk of an interaction. Another 26 Quercus species are predicted to host ten or more Agrilus species.

The model was not successful in predicting hosts of A. auroguttatus (goldspotted oakborer) in its introduced range in California.

black oak (Quercus kelloggii) in Cleveland National Forest killed by GSOB; photo by F.T. Campbell

It also predicted that few of China’s oak species might host Agrilus beetles. However, as Dr. Robert Haack notes (pers. comm. June 2026), larval hosts have been identified for only 13% of the nearly 1,200 Asian Agrilus.

Some Agrilus species have a very large number of predicted novel interactions. A. graminis and A. angustulus are predicted to have more than 40 novel oak hosts. Both have numerous known oak hosts; so their “polyphagous” nature is already documented.

Since two-thirds of 666 Agrilus species with known larval hosts exploit only one plant genus as a host in their native range, Hernández‐Gutiérrez, Nichols, and Kelly (2026) assert that they might spread faster if introduced to homogeneous rather than species-rich habitats. Dr. Haack believes that this statement is too broad (pers. comm. June 2026).

A. bilineatus; photo by Christina Butler via Wikimedia

Twolined chestnut borer

Haack and Blank (2024) document that the twolined chestnut borer, Agrilus bilineatus has preferentially infested apparently healthy English oak (Quercus robur) trees over healthy native oak trees in Michigan. In North America, A. bilineatus is a major pest of oaks and American chestnut (Castanea dentata)when they are stressed by drought or other factors. Infestation typically begins in the upper crown and proceeds downward; tree death often occurs within three years.

 At several sites in southern Michigan, where English oaks were intermixed with native white oaks (Quercus alba) and close to northern red oaks (Quercus rubra), A. bilineatus preferentially infested Q. robur trees that initially appeared healthy. Further study revealed that many of the English oaks attacked had low or depleted root starch levels.

Although these findings are cause for alarm, English oak is already used by 11 species of Agrilus in Europe. Perhaps the tree and ecosystem might have sufficient defenses in Europe. Meanwhile, A. bilineatus has been reported in Turkey as of 2018; I have found no recent information about the damage whether it is causing any damage there.

Data from Britain and Worldwide

Peyton et al. (2026) reviewed the effectiveness of a “horizon scanning” exercise conducted for Great Britain (England, Scotland and Wales). They report that 3,248 recognized non-native species have been detected in Great Britain, of which 2,016 have established self-sustaining populations. Some 194 (~10%) are considered invasive, that is, have negative impacts on biodiversity and wider ecosystem viability. These consist of 108 terrestrial species, 47 freshwater species, and 39 marine species. These bioinvaders cost the British economy an estimated ~£3.9 billion per year (the bulk of the damage is attributed to ash dieback, caused by the fungus Hymenoscyphus fraxineus).

In the decade between completion of the “horizon scan” and the present, 143 species were recorded as being introduced. The horizon scan predicted 31 of these species, 22%. Peyton et al. (2026) consider this to be success.

Peyton et al. (2026) report that globally, ~ 6% of non-native plant species are ranked as invasive. Among invertebrates, this proportion rises to 22%. Considering vertebrates introduced to Europe or North America, the figure is more than 50%!! I welcome global data that support my call for rethinking the “rule of tens” long relied on for estimating the proportion of non-native species that are invasive.  

Discussing bioinvaders’ role in causing extinctions, Peyton et al. (2026) report that 30 predators have been linked to declines and extinctions of 738 vertebrate species.

Peyton et al. (2026) also discuss the difficulty in predicting an introduced species’ impacts when in some cases the time lag between introduction and presence in the wild or between establishment and spread w/in the region can last decades or even a century. They cite as an example Senecio squalidus, which escaped the Oxford Botanic Gardens in the 1700s but started to spread only during mid-1900s.

Australia

More than 300 non-native insect pests, pathogens and nematodes have established on tree or shrub hosts in Australia; 20% have caused moderate to high impacts to commercial plantations, urban forests, or trees in natural ecosystems (Carnegie et al. 2026).The rate at which non-native forest pests and pathogens have been detected in Australia has doubled since 2018 compared to earlier decades: from ~ 1.5 to ~ 3 per year. Carnegie et al. (2026) attribute this rise to greatly expanded official surveillance efforts. Still, three-quarters of the most recent detections came too late for eradication to be attempted.

The Forestwatch program (inaugurated – under a different name – in 2022) includes pathogens. I rejoice!!! Still, the target species threaten primarily tree species not native to Australia but important to commercial forestry or urban forests: Asian longhorned beetle,  burnt pine longicorn (Arhopalus ferus), pine pitch canker, pine wilt disease, red turpentine beetle (Dendroctonus valens), Asian spongy moth, red needle cast, and sudden oak death. The exceptions are strains of Austropuccinia psidii not yet intro to Australia, and eucalypt leaf blight (caused by Teratosphaeria destructans) (Carnegie et al. 2026).

Austropuccinia psidii infection on Melaleuca in Australia; photo by John Tann via Flickr

Among the introduced pests causing the greatest damage to native species are

  • Phytophthora cinnamomi: this soil fungus can kill 40% of the plant species in the southern portion of Western Australia  – which is one of 36 “Biodiversity Hotspots” recognized by the Critical Ecosystem Partnership Fund.  
  • Austropuccinia psidii (cause of myrtle rust) in natural ecosystems; Members of the host family Myrtaceae occur in 11 of 13 major vegetation formations on Australia. Various authorities have identified 76 species as at risk to the rust.

I hope the Australians are developing strategies for landowners to counter damage by the polyphagous shot hole borer (Euwallacea fornicatus) and its associated fungus (Fusarium euwallaceae). DMF Outbreak detected near Perth, Western Australia, in 2021 – apparently three years after the actual introduction. By June 2025 authorities had determined that it was too widespread to be eradicated, so landowners will be responsible for any management.  (Carnegie et al. 2026) Impact is predicted to be greatest in urban landscapes, and cost up to AU$9.7 M per annum to manage.

Phytophthora pluvivora was first detected in Australia on an English oak, Quercus robur. However, it has since been recorded on native species in the Blue Mountains, including the critically endangered dwarf mountain pine (Pherosphaera fitzgeraldii) in a National Park.

SOURCES

Carnegie. A.J., B.A. Summerell, C. Trollip, F. Tovar, D.I. Smith, and J. McDonald. 2026. Sentinel trees for early detection of non-native forest pests and pathogens in Australia. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Haack, R.A. and R.B. Blank. 2025.  Susceptibility of English Oak (Quercus robur) to the Twolined Chestnut Borer, Agrilus bilineatus (Coleoptera: Buprestidae): Observations from Michigan. The Great Lakes Entomologist. 57: 113-125. https://doi.org/10.22543/0090-0222.2492

Hernández‐Gutiérrez, E., R.A. Nichols, and L.J. Kelly. 2026. Combined phylogenetic and geographic data can predict plant–pest interactions with high accuracy. New Phytologist (2026) doi: 10.1111/nph.71306

Peyton, J.M., S. Rorke, D.C. Aldridge, O.L. Pescott, K. Dehnen- Schmutz, D.G. Noble,  J. Sewell, A.J.A. Stewart,  T. Adriaens,  B.C. Beckmann,  J. R. Britton, J. Brodie1, P.M.J. Brown, I.C.N. Cavadino, P.F. Clark, A.M. Dunn, J.Foster, C. Harrower, M.C. Harvey, M.C. Jackson, T. Jones, C.A. Maggs, G. Martin, F. Mathews, A.C. Mill, D. Murphy,  E. Paganini, R. Payne, W. Rabitsch, T. Renals,    K. Schönrogge, R.H. Shaw, G.C. Smith, P.D. Stebbing, P.A. Stroh, H. Tidbury, E. Tricarico, J. Vallet,   K.J. Walker, L.E. Wood, C.A. Wood, B. Woodcock, H.E. Roy. 2026. Assessing the success of a horizon scanning approach in predicting invasive non- native species arrival. J Appl Ecol. 2026;63: https://doi.org/10.1111/1365-2664.70217

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
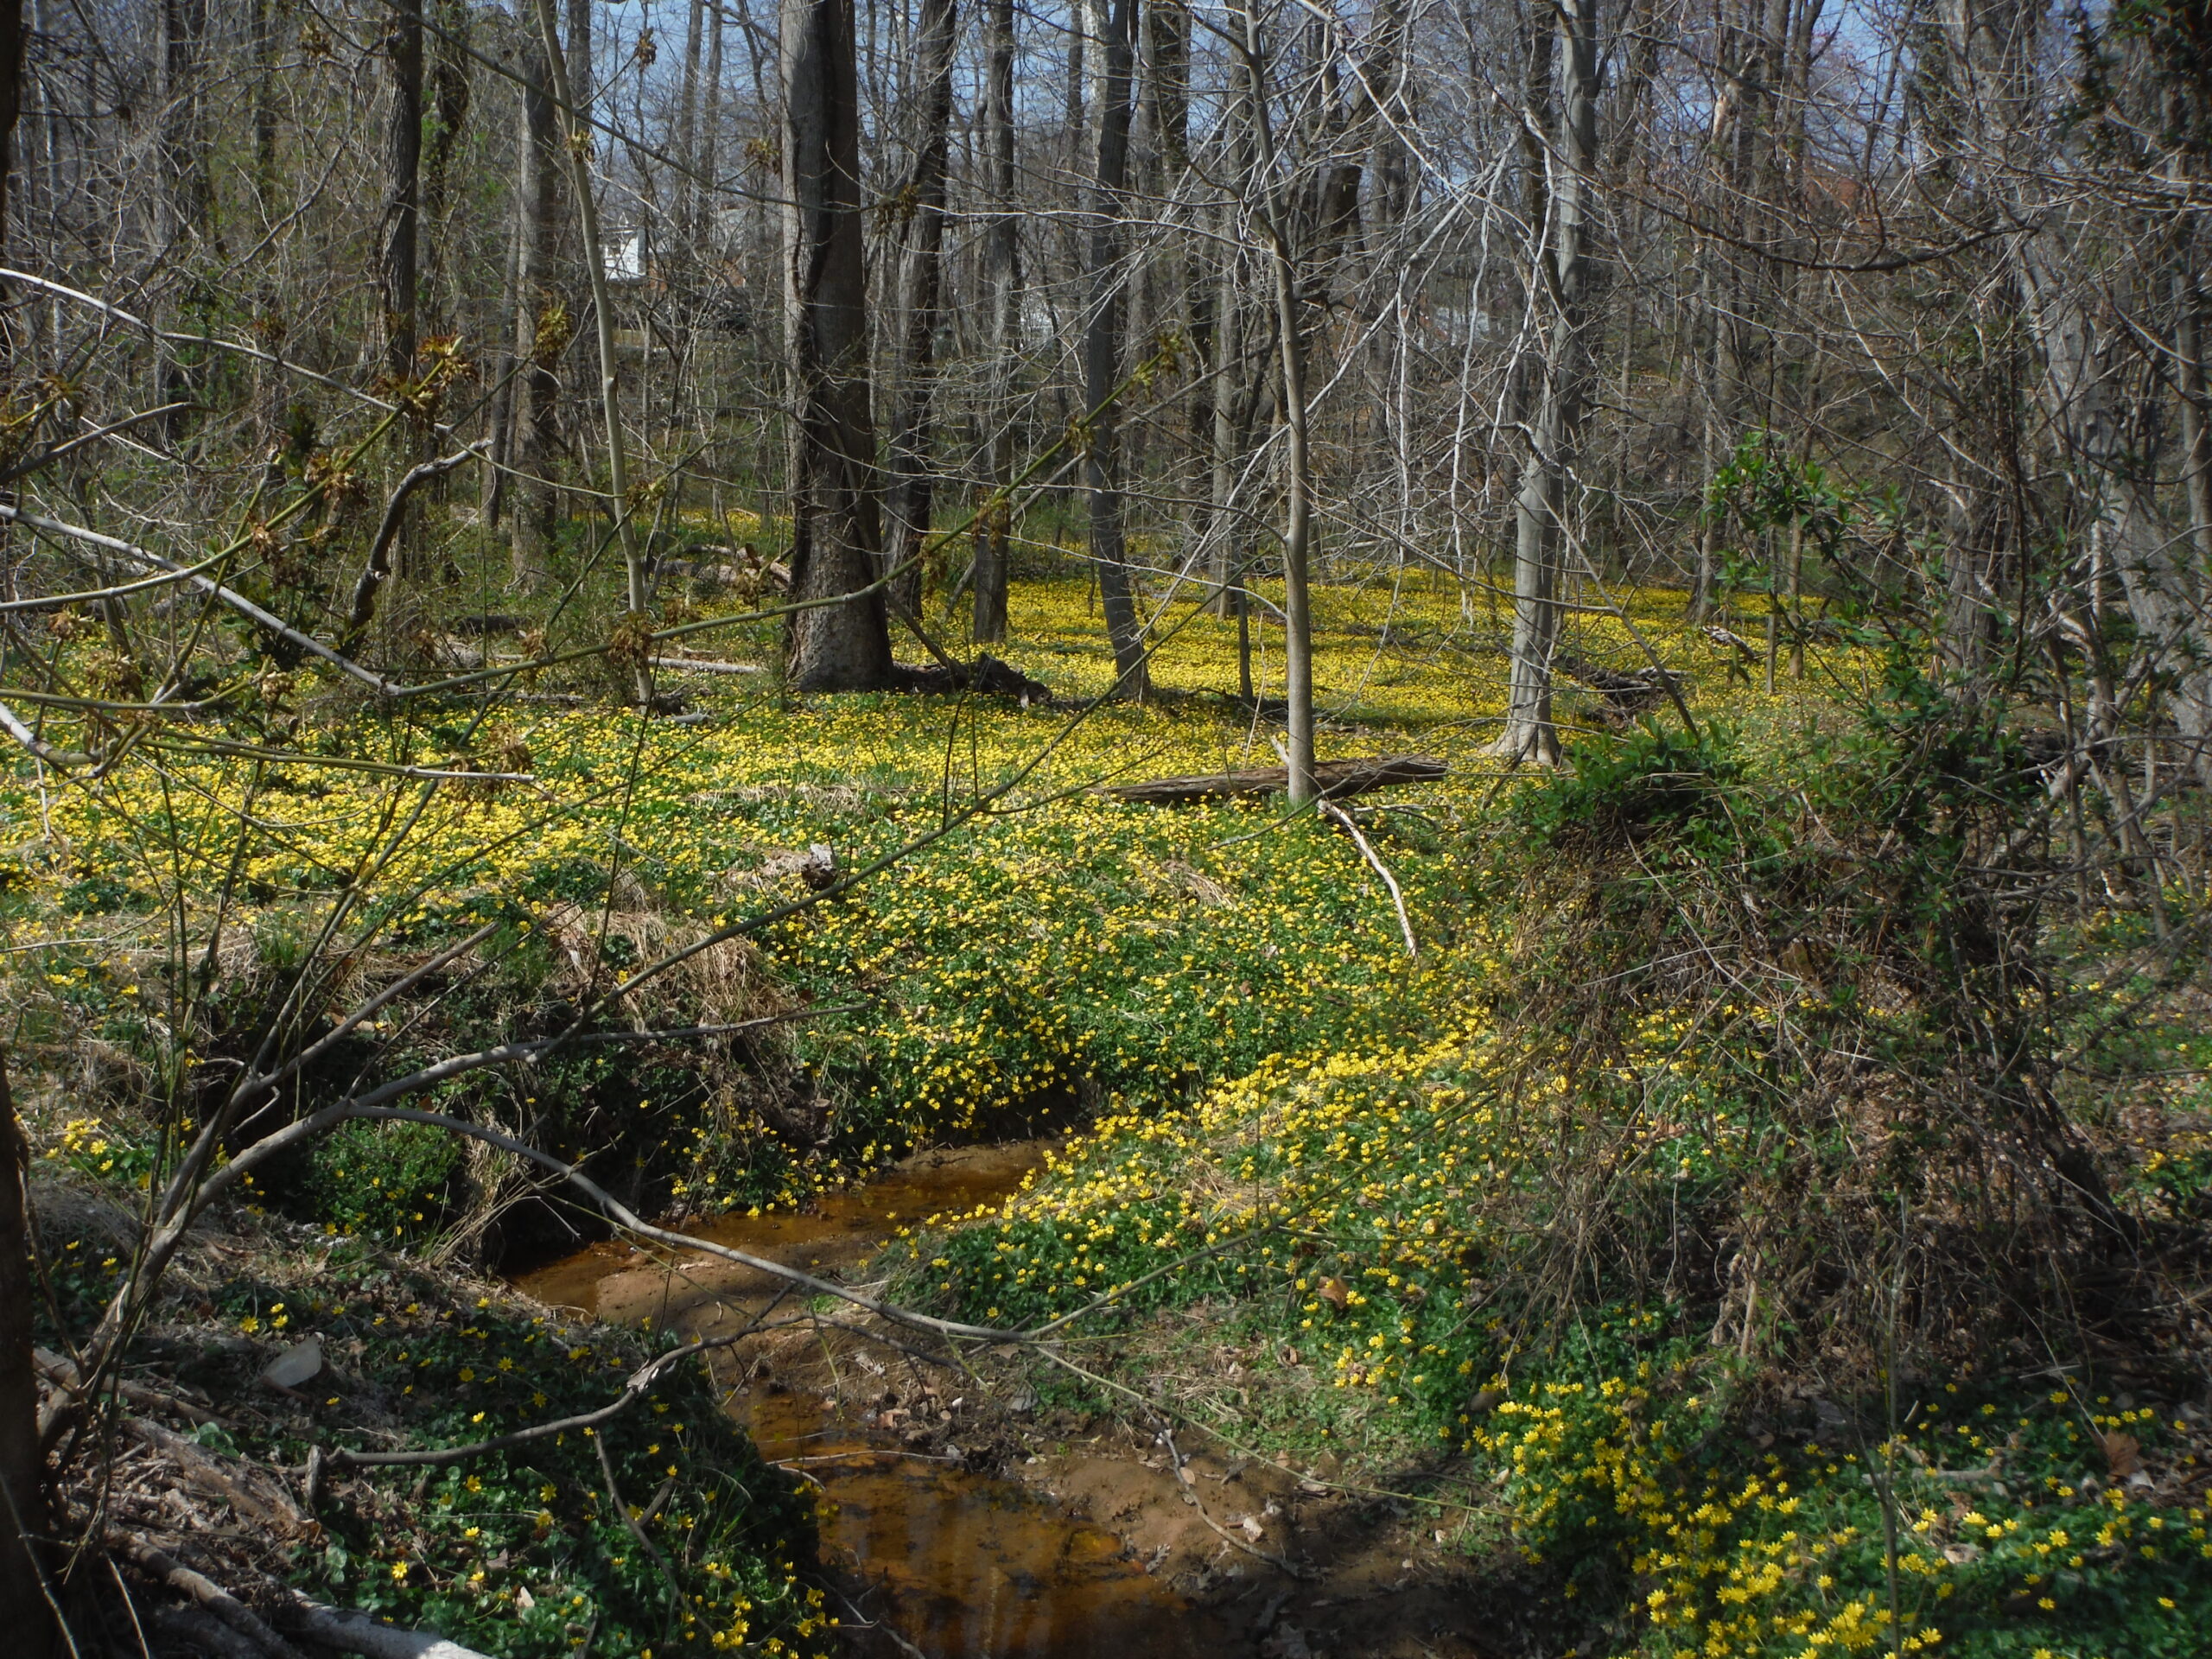
https://fadingforests.org

U.S. Imports from Asia rise … & as more regions expand ports, the pest risk spreads to new places

Pananax ship; photo by 2005emsaguinden via Wikimedia

Imports from Asia, specifically China, had surged in the first half of 2025 as importers tried to get ahead of new tariffs. Blog They then fell sharply, although there was also a shift in Asian suppliers from China to Vietnam and India. At the end of 2025, experts expected the slump to persist into 2026. However, now we learn that U.S. imports from Asia jumped 13% from April to May, to 1.68 million TEUs (Michael Angell, Journal of Commerce, June 16, 2026). According to Politico, the shift to importing goods from Vietnam, and to a lesser extent to Thailand and Indonesia, has continued.

American cities continue to compete for to build larger ports so they can receive more cargo. Of course, more cargo means more incoming containers. As my blogs document (click “wood packaging” in the “Categories” section below the “Archives”), containers and especially the crates and pallets inside them too often transport wood-boring insects and other invasive species.

My source of information on these developments is from the Journal of Commerce website. Unfortunately, access is blocked by a paywall.

Recent reports concern port cities dredging and widening their ports in hope of attracting increased import volumes.

Norfolk; photo by PghPhxNfK via Wikimedia

Norfolk, Virginia

This month the Virginia Port Authority (VPA), Governor Abigail Spanberger and other federal, state, and local officials inaugurated the Port of Norfolk’s expanded capacity. At 55 feet, Norfolk is now the deepest and widest port along the East Coast. The project, begun in 2019, will allow Norfolk to handle vessels carrying up to 18,000 TEUs [twenty-foot equivalent containers]. Authorities are encouraging ocean carriers to call there.

The port was visited by 1,497 container ships over the past 12 months; nearly a quarter had a capacity greater than 11,000 TEUs.

Virginia’s container volumes grew on average 3% annually between 2017 and 2024. In 2025, total container volume fell 8% from 2024 because shippers hoped to avoid tariff deadlines by unloading cargo at a first or second port of call. Virginia was the six-busiest US port for imports this year through May, handling 635,205 TEUs. That was up 2.6% from the same five-month period a year ago. To attract shippers to Norfolk as a first or even second port of call for more container services, Virginia Port Authority CEO Sarah McCoy said, Virginia needs to emphasize rail links. This involves expanding the region’s distribution center network.

The project to dredge and widen the port began in 2019. The total project has a budget of $1.4 billion. The project included adding two ultra-large container vessel (ULCV) berths at each of its two container terminals. The final component is to renovate the North Berth, including developing a fifth ULCV berth, plus four new ship-to-shore cranes and semi-automated stacking cranes in its container yard. Completion is scheduled for mid-2027. At that time, the port’s total handling will reach 5.8 million TEUs. The International Longshoremen’s Association (ILA) is contesting installation of semi-automated stacking cranes in a series of lawsuits.

Other East Coast ports are also adding terminal capacity. This includes the Port of Baltimore, where a shipping company is developing a container terminal that includes handling two ULCVs simultaneously. Apparently they are not deterred by the months-long closure of the Port of Baltimore caused by a ship colliding with a bridge downstream from the port.  

[Information from Michael Angell, Senior Editor, East Coast Ports. “Norfolk aims to be preferred USEC gateway with deeper port” June 18, 2026]

U.S. Army Corps of Engineers dredge in the Savannah River

The Port of Savannah remains dominant. In 2025 Savannah and the roll on-roll of facility in Brunswick together handled nearly 5.7 million TEUs, an increase of 2.6% or 146,000 TEUs compared to 2024. Even so, Georgia Ports is financing a $4.5 billion port and inland infrastructure plan which will add five new container berths in Savannah, the most new berths of any U.S. port and one new RoRo berth in Brunswick. Port officials brag about their rapid turnover of cargo from ship to rail. Forty-two double-stack trains per week take this cargo to Atlanta, Memphis, Nashville, Charlotte and Orlando. The Port Authority also operates two inland terminals – in in Chatsworth and Gainesville, Ga.

Corpus Christi

As I have reported in previous blogs, Gulf Coast ports are also upgrading to receive more shipments. DP World, a Dubai-based terminal operator, is negotiating to develop a container terminal at the Port of Corpus Christi. This would open this port to container logistics.

Corpus Christi is already the third-busiest port in the US by gross tonnage, behind Houston and South Louisiana. The bulk of cargo is petroleum and bulk commodities. (In past years, dunnage associated with bulk commodities proved to cause pest-infestation problems in nearby Houston.)

dunnage piled on the dock at Houston; photo by S. Useman

Last year Corpus Christi completed an eight-year, $625 million project to widen and deepen its main shipping channel (from 47 feet to 54 feet). The expansion allows visits by super-post-Panamax container vessels.

[Information from Michael Angell, Senior Editor, East Coast Ports. “DP World begins talks with Corpus Christi for container terminal project” June 16, 2026]

Warehouse Capacity

Leaders of logistics managers note that importers and domestic manufacturers are diversifying their supply chains – both warehouse facilities and shipping routes – because of ongoing supply chain disruptions even years after COVID 19. While many industrial warehouses across the U.S. still have vacancies (averaging above 7%), some markets are filling up. They mention Chicago, Indianapolis, Memphis, Dallas, and Kansas City. These cities’ warehouse vacancies average ~5%. Indianapolis leads; asking rents for industrial space there have climbed more than 50% over the past five years. Phoenix also anticipates increased demand for space, although its current vacancy rate is 10.6% – the highest vacancy rate of the 25 largest markets.

The move away from Los Angeles-Long Beach began years ago. To move freight inland, shippers need options, particularly access to intermodal rail.

shipping containers at Long Beach in the early 2000s; photo courtesy of Bob Kanter of the Port of Long Beach

The experts attribute this growth to the need for more flexibile supply chains and demand for materials used in constructing data centers. Demand for the second category is reportedly strongest in the Southeast, followed by interior central markets.

[Information from William B. Cassidy, Senior Editor, Trucking. “US warehousing expanding faster at key inland hubs” June 18, 2026]

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
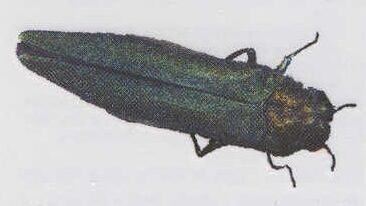
https://fadingforests.org

Bioinvader Threat to Caribbean cacti – Who is Protecting Them?
Photo of infested cactus at Cabo Rojo National Wildlife Refuge, Puerto Rico. Taken August 20, 2018 by Yorelyz Rodríguez-Reyes

For 15 years I have maintained a profile of the Harrisia cactus mealybug Hypogeococcus pungens because it threatens columnar cacti in the subfamily Cactoideae from the Caribbean basin and possibly in the American Southwest and Mexico. My recent attempts to clarify the current situation have been frustrated by the apparent collapse of funding support for scientists trying to conserve these cactus species.

The dry regions of the Caribbean Islands are home to about 100 native cacti, 75% of which are endemic. According to the Center for Plant Conservation, 20 species are listed as threatened by the IUCN. Puerto Rico specifically is home to 14 cactus species, at least three of which are endemic.

How and when the mealybug first invaded the Caribbean and North America is unknown. The presence of the insect now known as H. pungens Hyp-C on Puerto Rico was detected in the Guánica Commonwealth Forest and Biosphere Reserve on the island’s southern coast in 2005 (Zimmerman et al. 2010). However, the actual introduction probably occurred about ten years earlier, in about 1996 (Poveda-Martinez et al. 2022).  See map of locations below.

In the 20 years since then, the mealybug has spread across the island’s dry districts. By 2010, it was estimated to be present on about 1,400 km2. By 2014 – nine years after detection — the mealybug had reached the small island of Caja de Muertos. The most recent survey of which I am aware (date unclear) detected the mealybug on 268 out of 445 cactus plants examined (60%) in 12 out of 39 sites examined (Poveda-Martinez et al. 2022). The mealybug is also killing native cacti on the nearby U.S. Virgin Islands (Poland et al. 2019), although I have found no data on this invasion or its impact.

Below – columnar cacti on St. John, US Virgin Islands; photos by F.T. Campbell

H. pungens Hyp‑C threatens seven of 14 native cactus species in Puerto Rico. Three of the cacti are endemic; two are federally listed as endangered species: Harrisia portoricensis and Leptocereus grantianus (USDA ARS). Since the mealybug’s detection in Puerto Rico, it has caused extensive damage to Pilosocereus royenii (Royen’s tree cactus), Leptocereus qaudricostatus (pitaya), Melocactus intortus (turk’s cap), and an introduced cultivar, Cereus hexagonus. It has caused minor damage to Stenocereus fimbriatus (Zimmerman et al. 2010). These cacti provide food or shelter for endemic bats, birds, moths and other pollinators (Segarra and Ramirez; USDA ARS).

The insect’s attack promotes abnormal gall-like growth on the stem and deformed flowers. These deformations severely affect infested plants’ reproduction and eventually survival (Poveda-Martinez et al. 2022).

Biological Control

When the mealybug was first detected Commonwealth and federal agencies tried to counter it. A search for possible biocontrol agents in the insect’s native range in Argentina began the 2010. While no funds have ever been appropriated for this activity, for several years the U.S. Department of Agriculture supported the work by allocating funds to the Agriculture Research Service Insect Behavior and Biocontrol laboratory in Gainesville, Florida, from broader programs. Dr. Stephen Hight took the lead, working with colleagues in South America. According to Dr. Hilda Diaz-Soltero, then a USDA official, these funds came primarily from the USDA Invasive Species Coordination Program and APHIS Eastern Region. In fiscal years 2017 and 2019, an additional ~$550,000 came in the form of grants under APHIS’ Plant Pest and Disease Management and Disaster Prevention Program. Link Scientists at the Center for Excellence in Quarantine and Invasive Species at the University of Puerto Rico devoted at least a decade to the search.

Scientists focused on two parasitoid wasps, Anagyrus cachamai and A. lapachosus (Hymenoptera: Encyrtidae). A third candidate, the predator Hyperaspis conclusa, was also assessed (Aguire et al.).

Research on the mealybug-wasps interaction uncovered troubling patterns. First, it has long been known that some mealybugs believed to be belong to the species Hypogeococcus pungens feed on columnar cacti while others feed on plants in two unrelated families, Amaranthaceae and Portulacaceae (USDA ARS; Zimmerman et al. 2010). Would the introduced wasps attack the cactus-feeding mealybug in sufficient numbers?

The confusion over how many mealybug species have been introduced – and where – severely hampered development of a program. (The mealybug has been introduced to control invasive cactus in Australia and South Africa. Most sources say it has been highly effective – prompting the initial concern when it appeared on Puerto Rico.) I have been unable to find any information about the status of the candidate biocontrol agents more recent than 2022.

Genetic Conservation

The USDA also partnered with the Naples (Florida) Botanical Garden to collect fruits and vegetative material for ex situ conservation. Rigorous phytosanitary procedures were followed to ensure the absence of the mealybug. Collections of fruits and vegetative material provided 1,298 cacti samples from 13 species, representing 1,173 maternal lines from 91 sites throughout Puerto Rico. A total of 90,720 seeds representing 8 species are banked at the NBG for long-term storage. Propagation of the vegetative material has 56% success, and plants are incorporated into the NBG’s living collections. (These figures include Opuntia cacti that are hosts of a second invasive insect, Cactoblastis cactorum.)  

Genetic Concerns

Scientists now consider Hypogeococcus pungens (Hemiptera: Pseudococcidae) to be a species complex composed of at least five putative species. The species are separated in part by the plants they use as hosts. Two of the complex have apparently been introduced to Puerto Rico: H. pungens Hyp‑C feeds on cacti; H. pungens Hyp‑AP feeds on hosts in the Portulacaceae & Amaranthaceae. Both evolved from putative source populations in Brazil (Poveda-Martinez et al. 2022).

The two species H. pungens Hyp-C and Hyp-AP are currently separated on Puerto Rico by host preferences and climatic niches. They also occupy different geographic areas. Scientists fear that ongoing climate change could allow H. pungens Hyp-C to establish farther into the island’s interior and in a large area in the north. Such range expansion would end the geographic separation. Overlapping of the two species is likely to exacerbate the threat to Puerto Rico’s cacti. Most directly, it would complicate implementation of management strategies, especially biological control. Intermixing of the two species could also facilitate hybridization which might result in more vigorous attacks or a broadened host range. Hybridization is frequent in closely related species (Poveda-Martinez et al. 2022).

The Mealybug is Frequently Introduced

Mealybugs that feed on cacti and believed to be in the species Hypogeococcus pungens made multiple appearances in southern California between 2000 and 2018 – in gardens and in nurseries. Confusingly, CDFA reports interception of the mealybug on alternanthera and ludwigia plants shipped from Florida (CDFA 2018). I have no more recent data. The population in Florida was reported to be present in 16 counties in 2009); it might be the species that feeds on plants other than cacti (Poveda-Martinez et al. 2022). Other populations has been reported in the Dominican Republic (no date) (CDFA 2018); and in Hawai`i in 2005 (Hawaii Department of Agriculture new pest report). A mealybug that feeds on Amaranthaceae and Portulacaceae was detected in 2000 in San Juan, Puerto Rico (Poveda-Martinez et al. 2022).

In the absence of control measures, scientists expect H. pungens Hyp-C to continue decimating Puerto Rican cactus diversity and threaten other cactus rich ecosystems across the Caribbean islands, Central America and, potentially, North America (Poveda-Martinez et al. 2022).

saguaro and organ pipe cacti in Organ Pipe Cactus National Monument; photo by F.T. Campbell

North America has more than 500 columnar cactus species in the Cactoideae (Zimmerman et al. 2010). Some of these cacti are already endangered, e.g., several Pediocactus. Others are totems of the desert, e.g., the saguaro (Carnegiea gigantea) and organ pipe (Stenocereus thurberi) cacti. Picture The larger ones, particularly, play important ecological roles. It is not known how vulnerable individual species are to the mealybug (Golubov pers. comm. January 2011). In Mexico several mealybugs in the same genus are already present. The natural enemies of these mealybugs might be able to attack H. pungens Hyp-C if it invades the country (Zimmerman et al. 2010). Despite the well-founded concern, apparently no funds have been allocated by governments or conservation organizations to studying the vulnerability of these cacti to one or more mealybugs in the Hypogeococcus genus.

The most likely pathway by which the mealybug is spread is the trade in plants for planting (the horticultural trade) (Zimmerman et al. 2010). A decade ago APHIS reported intercepting mealybugs on cactus (primarily on roots) imported from Germany, Peru, and Puerto Rico. APHIS has also intercepted several other mealybugs in the same genus – on plants (including orchids and bromeliads as well as cacti) from Belize, Costa Rica, Ecuador, Guatemala, Honduras, Mexico, Panama, Peru, and Venezuela (USDA APHIS alert).

A decade ago NatureServe and IUCN found that 31% of Earth’s cactus species were threatened with extinction. They named overharvesting (often for the illegal horticultural trade) and destruction of habitat by smallholder livestock ranching and farming. Did not mention predation by introduced insects – although that is now manifest not only in the cactus mealybug but also the cactus moth.

Sources

Aguirre, M. G. Logarzo, S. Triapitsyn, H. Diaz-Soltero, S. Hight, O. Bruzzone. 2023? Effect of egg production dynamics on the functional response of parasitoids

California Plant Pest and Disease Report. 2005. Vol. 22 No. 1. Covering Period from July 2002 through July 2005.California Department of Food and Agriculture. 2018.California Pest Rating for Hypogeococcus pungens Granara de Willink | Harrisia cactus mealybug Hemiptera: Pseudococcidae Pest Rating: A California Pest Rating for Hypogeococcus pungens Granara de Willink | Harrisia cactus mealybug Hemiptera: Pseudococcidae Pest Rating: A

Hawaii Department of Agriculture. 2006. https://hawaii.gov/hdoa/pi/ppc/2006-annual-report/new-pest-detections  (accessed 11/1/10)

Poland, T.M., Patel-Weynand, T., Finch, D., Miniat, C. F., and Lopez, V. (Eds) (2019), Invasive Species in Forests and Grasslands of the United States: A Comprehensive Science Synthesis for the United States Forest Sector.  Springer Verlag.

Poveda-Martinez, D. N.A. Salinas, M. Belen Aguirre, A.F. Sanchez-Restrepo, S. Hight, H. Diaz-Soltero, G. Logarzo,  and E. Hasson. 2022 Geonomic & ecol evidence shed light on the recent demographic history of two related invasive insects. Scientific Reports.

Segarra-Carmona, A.E., A. Ramirez-Lluch. No date. Hypogeococcus pungens (Hemiptera: Pseudococcidae): A new threat to biodiversity in fragile dry tropical forests.

Segarra-Carmona, A.E., A. Ramírez-Lluch, I. Cabrera-Asencio and A.N. Jiménez-López. 2010. First Report of a New Invasive Mealybug, the Harrisia Cactus mealybug Hypogeococcus pungens (Hemiptera: Pseudococcidae). J. Agrie. Univ. RR. 94(1-2):183-187 (2010)

Srivastava, M., P. Srivastava,  R. Karan, A. Jeyaprakash, L. Whilby, E. Rohrig, A.C. Howe,  S.D. Hight, and L. Varone. 2019. Molecular detection method developed to track the koinobiont larval parasitoid Apanteles opuntiarum (Hymenoptera: Braconidae) imported from Argentina to control Cactoblastis cactorum (Lepidoptera: Pyralidae). Florida Entomologist 102(2): 329-335.

Triapitsyn, Aguirre, Logarzo, Hight, Ciomperlik, Rugman-Jones, Rodriguez. 2018. Complex of primary and secondary parasitoids (Hymenoptera: Encyrtidae and Signiphoridae) of Hypogeococcus species. mealybugs (Hemiptera: Pseudococcidae) in the New World. Florida Entomologist Volume 101, No. 3 411

USDA Agriculture Research Service, Research Project: Biological Control of the Harrisia Cactus Mealybug, Hypogeococcus pungens (Hemiptera:pseudococcidae) in Puerto Rico Project Number: 0211-22000-006-10 Project Type: Reimbursable

Zimmermann, H.G., M.P.S. Cuen, M.C. Mandujano, and J. Golubov. 2010. The South American mealybug that threatens North American cacti. Cactus and Succulent Journal. 2010 Volume 82 Number 3