Confirmation of failures of the international phytosanitary system

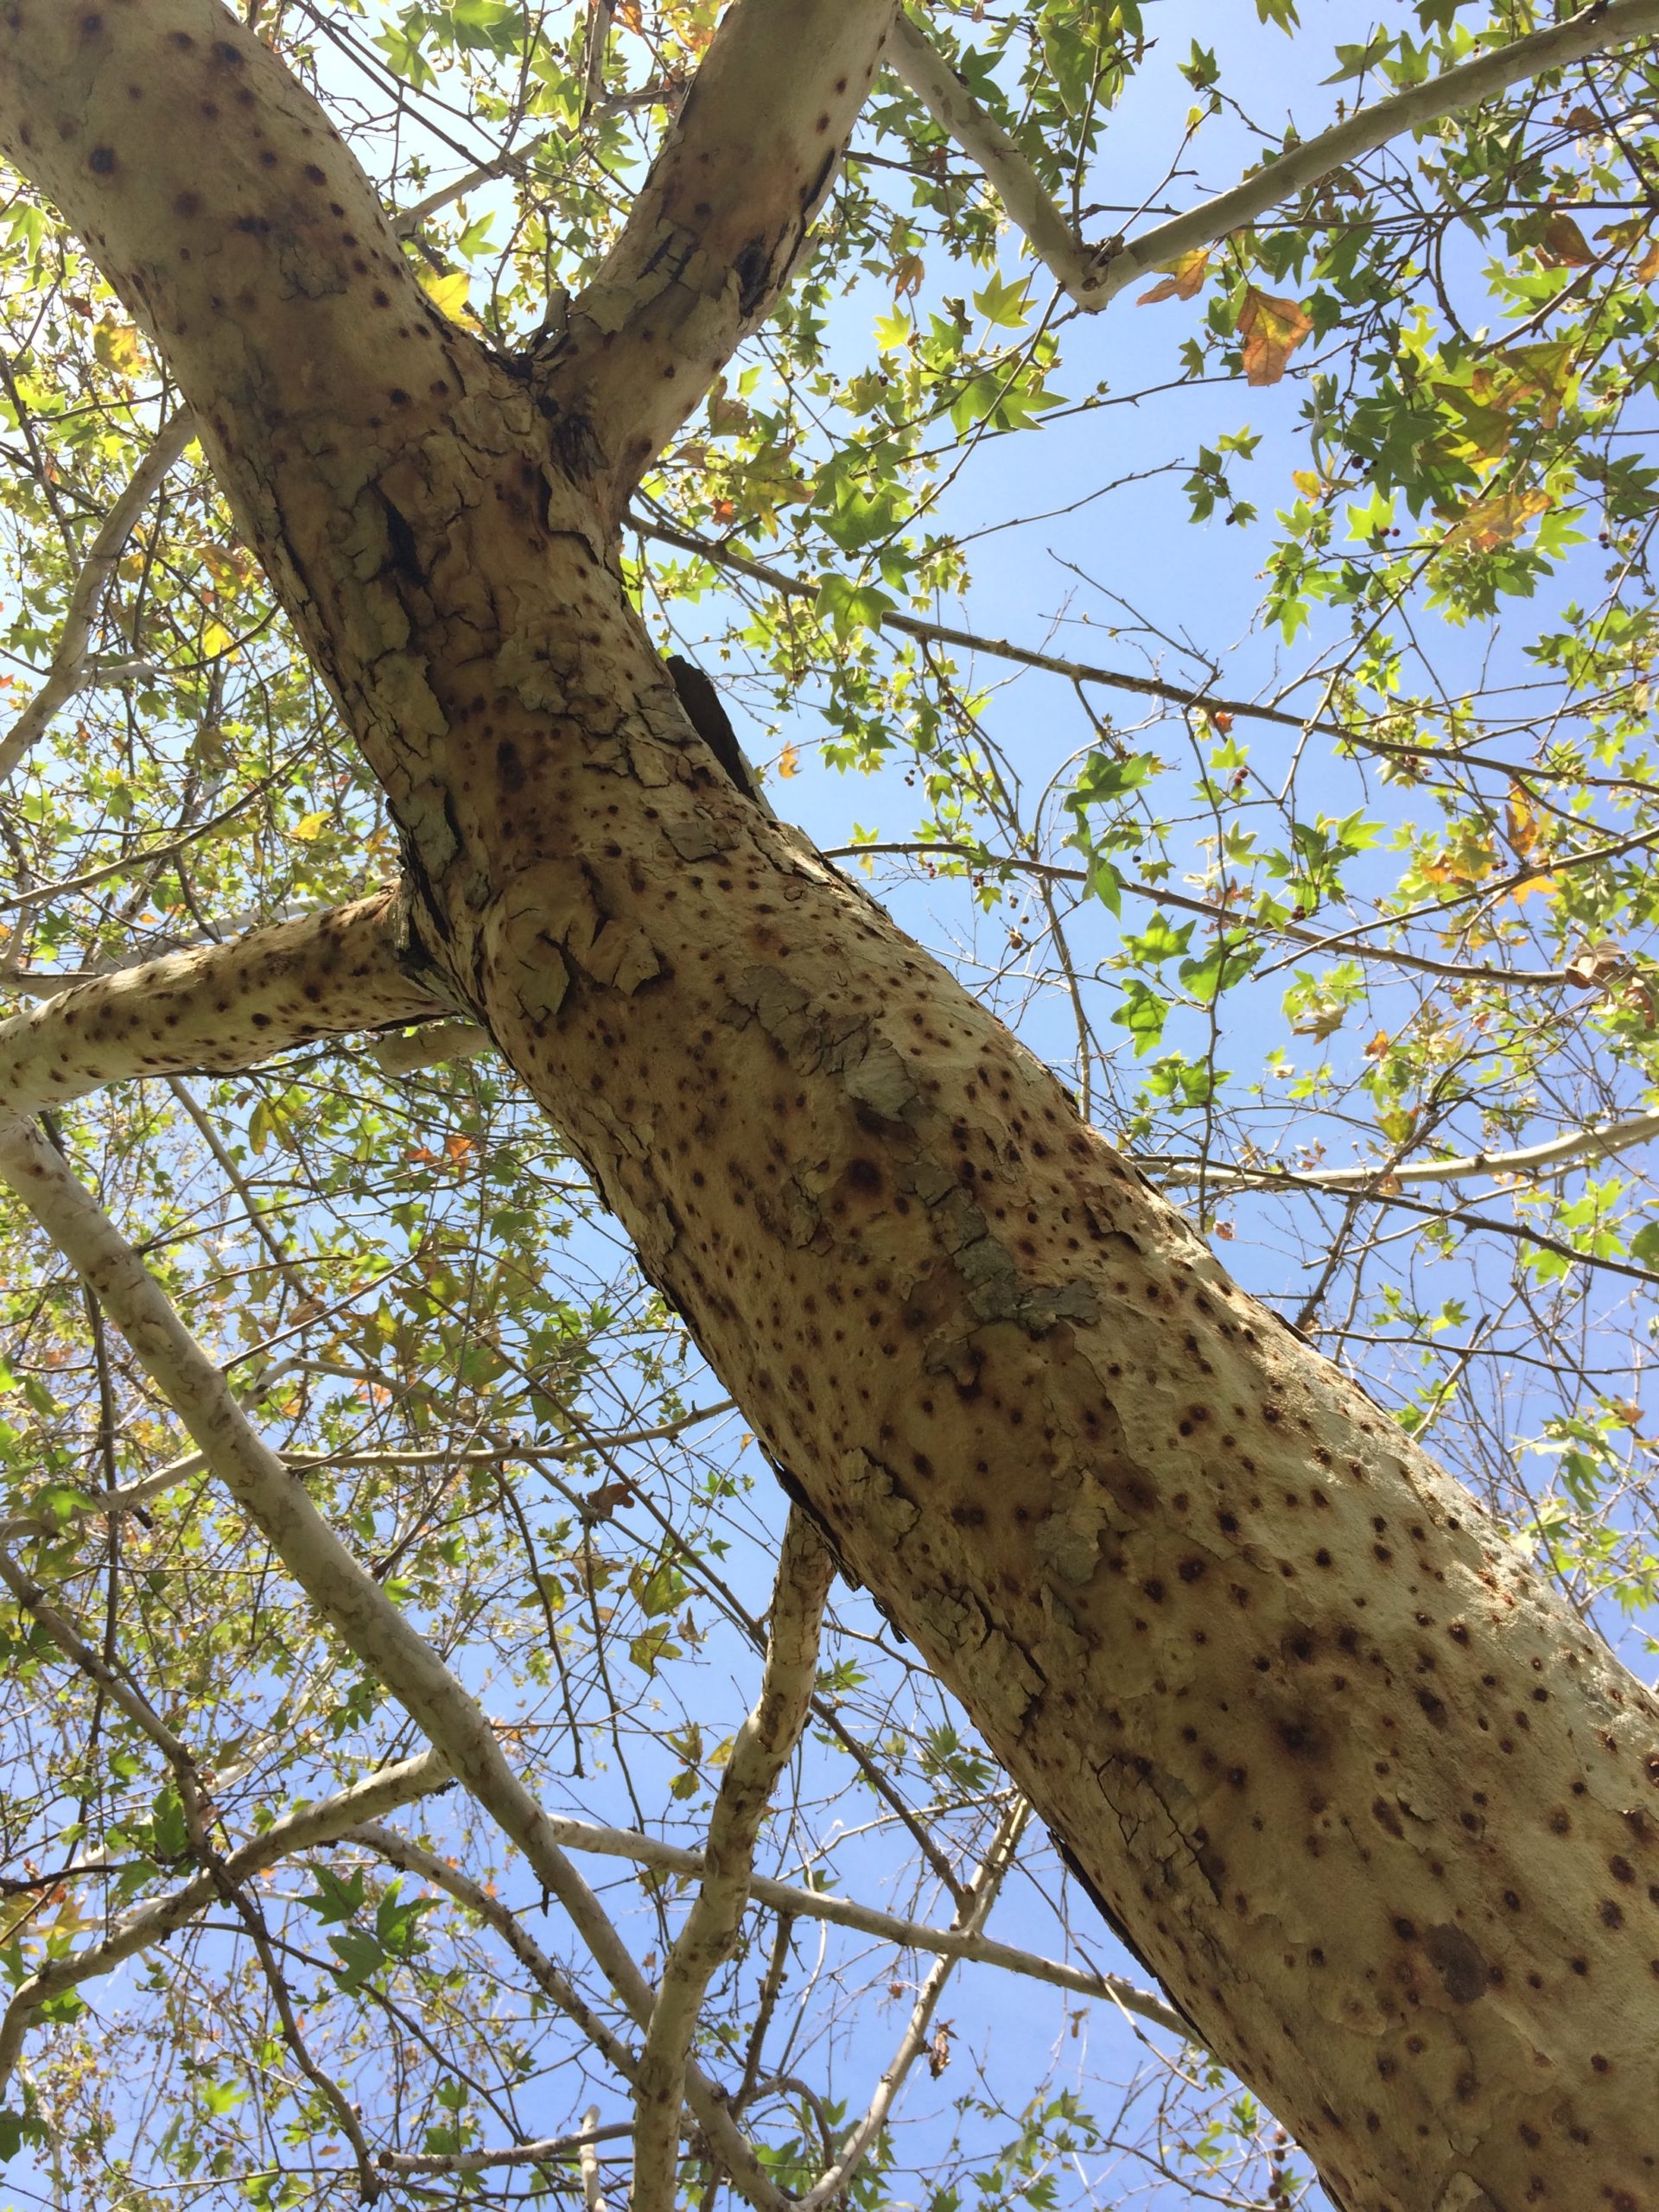
California sycamore infested by PSHB; photo by Bea Nobua

Lantschner et al. (2026; full citations at the end of this blog) review global spread of an ambrosia beetle species complex, the polyphagous shot hole borer (PSHB, Euwallacea fornicatus). This complex has caused significant damage in southern California and is now poised to raze unique plant communities in South Africa, Western Australia, and possibly elsewhere. Dell, Xu, and Chi (2026) say that introductions of these species pose serious challenges to global biosecurity programs and forest health management.

Unfortunately, neither Lantschner and colleagues nor Dell, Xu, and Chi, nor even Pennisi’s summary of the situation in Science (2026) suggests the kind of bold changes to the international phytosanitary system needed to prevent repetitions of this disaster.

Ambrosia beetles are especially suitable study subjects for analyzing international movement of non-native species. Some reasons result from the beetle’s biology: they have broad host ranges, close associations with pathogenic fungal symbionts, cryptic biology, specialized breeding systems which allow extremely low populations to start an infestation, and the ability to establish across diverse climatic regions. Other reasons stem from the beetles’ frequent association with international trade in timber and/or ornamental plants.

PSHB’s Impact in California

California has been invaded by three species of Euwallacea — Euwallacea fornicatus s.s., Euwallacea kuroshio, and Euwallacea interjectus. The beetles vector three previously undescribed species of fungus that cause disease in host trees: Fusarium euwallacea, Fusarium kuroshium, and Fusarium floridanum.

Euwallacea fornicatus s.s. (polyphagous shot hole borer, or PSHB) came to attention in late winter 2012, when a new insect/pathogen complex was discovered causing damage to avocado trees in residential neighborhoods and a commercial avocado grove in Los Angeles County, California. Later studies determined that the beetle and its associated fungus had been in California since at least 2003 (Eskalen et al. 2013).

Over the nearly 15 years since its discovery, the PHSB/pathogen complex has spread across much of southern California. Populations are established in Orange, San Diego, Los Angeles, Riverside, San Bernardino, Ventura and Santa Barbara counties.   The separately introduced species Kuroshio shot hole borer (KSHB) was discovered in late 2013 in San Diego County. It has since spread to Mexico. Californians now track the two species as one; a map showing their current known distribution is posted here.
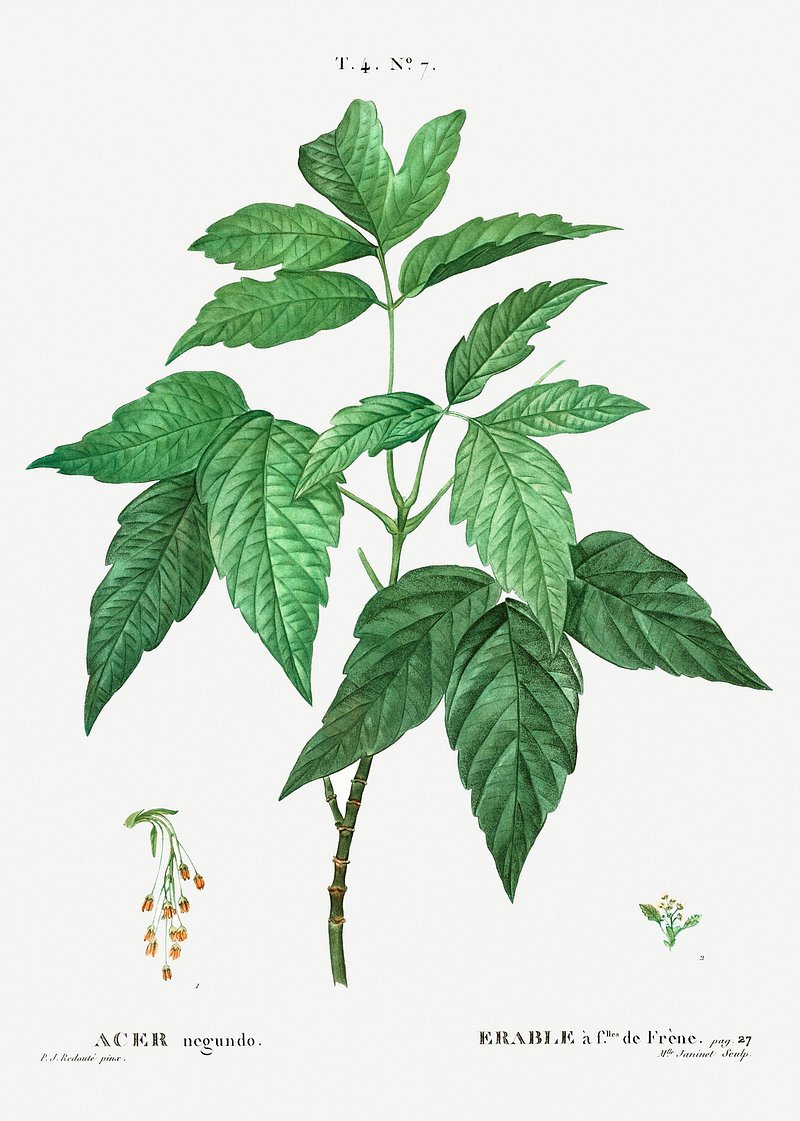
Box elder (Acer negundo) from Traité des Arbres et Arbustes que l’on cultive en France en pleine terre (1801–1819) by Pierre-Joseph Redouté. Original from the New York Public Library. Digitally enhanced by rawpixel.

Certainly a wide range of tree species face a challenge – as do their associated natural or anthropogenic systems. Nearly 600 plant species in more than 30 plant families are known hosts of PSHB worldwide (Ceriani-Nakamurakare, Johnson and Gomez, 2023). In southern California specifically, 65 woody species are able to support reproduction of both the beetle and the pathogen. The preferred and most susceptible hosts are several species in the maple (Acer), Parkinsonia, plane (Platanus), oak (Quercus), and willow (Salix) genera. Box elder (A. negundo) is so susceptible that it is considered a sentinel tree. The following additional native species are also hosts: big leaf maple (Acer macrophyllum); California sycamore (Platanus racemose); three Populus species, P. fremontii (Fremont cottonwood), P. nigra (black poplar), and P. trichocarpa (black cottonwood); Valley oak (Quercus lobata); and three willows – black (Salix gooddingii), red (S. laevigata) and arroyo (S. lasiolepis). Three more oaks – coast live oak (Q. agrifolia), canyon live oak (Q. chrysolepis), and Englemann (Q. engelmannii) – are less susceptible; they suffer branch dieback rather than death.

Given PSHB’s wide host range, it is not surprising that Lynch et al. (2025) found that regions at risk of future invasion are determined largely by climate rather than host abundance. Areas where temperatures are sufficiently warm to allow the beetle to pass through at least five generations per year include parts of southern California, drier regions of the San Francisco region, and portions of the Central Valley. A risk map for California is available here.

The E. fornicatus and E. kurosio combined outbreak has killed large numbers of trees in southern California’s coastal counties – although I have been unable to find an estimate.  Meanwhile,  additional outbreaks have been detected. The PSHB was found in the San Jose area in 2023. This location is close to the state’s Central Valley – where vulnerable almond, pistachio, and other crops grow (Pennisi, 2026). A third, related species, E. interjectus, also turned up. See a map of distribution of all three Euwallaceae established in California here.

A dozen years after their presence was detected, Dr. John Kabashima led a lobbying effort that persuaded the state legislature to fund a collaborative program comprising an action plan, five research initiatives, and a comprehensive outreach and education strategy across the state (Dell, Xu, and Chi). These funds ran out at the end of 2025, while the infestation continues.

As of the first half of 2026, official monitoring projects were reported to be under way in four of the seven invaded counties, Los Angeles, Orange, Riverside, and San Bernardino. This effort is now being cut back because state funding supporting it has expired. For example, Los Angeles County carried out surveys in 240 parks in 2025, but planned to survey only 146 in 2026. While in most parks the infestations were described as light or moderate, five parks with heavy infestations were detected in 2025; trees in a sixth park were reported to be recovering.

Attention continues from the California Invasive Species Advisory Committee, Los Angeles and Orange County Master Gardeners Emerging Tree Pests Groups, University of California Agriculture and Natural Resources (UC ANR) representatives, UC Cooperative Extension from various counties, and Cal-Fire. These organizations seize opportunities to educate the public about the shot hole borers’ impacts. 

Dr. Paul Rugman-Jones of the UC Riverside Department of Entomology is studying possible biocontrol agents. In early 2026 he was working w/ APHIS to set up research colony of Phymastichus nudusdraco, a wasp native to Taiwan that parasitizes PSHB there. He and a postdoc continues surveys on that island and elsewhere in Southeast Asia. Dr. Rugman-Jones is also searching for potential natural enemies already established in southern California.

From Asia to a World-wide Pest

The polyphagous shot hole borer has been detected in nine countries on five continents since 2000 (Lantschner et al. 2026). Many of these introductions have occurred since stricter biosecurity measures, i.e., International Standard of Phytosanitary Measures #15, came into force with the purpose of reducing introductions of insects associated with wood packaging material.

By combining data on the distribution of the species’ 36 haplotypes, phylogenetic relationships and dates of first detections, Lantschner et al. (2026) have identified seven independent introduction events of E. fornicatus: to the continental United States, Hawai`i, South America, Central Europe, Spain, Türkiye, and South Africa. I am unsure why this list does not include the introduction to Israel, detected in 2009.  

Lantschner et al. (2026) suggest two contradictory explanations for this explosive spread. On one hand, beetle populations in the species’ native Asian range might have increased recently. On the other, higher trade volumes from these countries have opened new pathways for transport. I favor the second explanation since exports from China have risen from less than $500 billion in 2003 to approximately $4 trillion in 2025. Exports from Vietnam rose from about $22 billion to $500 billion over the same period.  
Lantschner and colleagues compare the PSHB’s range of introduced populations to the more restricted locations invaded by another species in the genus, E. perbrevis. They believe that the latter is more restricted to humid tropical regions. It has been introduced to several islands in Oceania, and possibly northern Australia (Queensland). Many of these countries might be less active in global trade than the countries to which PSHB has been introduced. This shield is shrinking, however, as more countries expand their trade. Lantschner et al. (2026) warn that E. perbrevis’ establishment in subtropical FL and Panama indicates it might also tolerate broader climatic conditions than previously assumed. They think that E. perbrevis populations established in Central America might expand into northern South America, including the Amazon basin and the Brazilian coast. Another area at risk is central Africa.

Neither Lantschner et al. (2026) nor Dell, Xu, and Chi (2026) discuss why other species in the genus have been introduced to fewer locations. Euwallacea kurosio and E. interjectus are also established in California, but nowhere else.  

PSHB Threatens Severe Impacts in its Introduced Ranges Other Than California

The outbreak in South Africa occupies the largest geographic region of any PSHB outbreak on Earth (Bierman, Roets, and Terblanche 2022). Dell, Xu, and Chi (2026) anticipate significant economic costs tied to the need to remove affected urban trees. The article in Science (Pennisi 2026) quotes Stellenbosch University ecologist Francois Roets as saying the long-term consequences of these forest invasions will be “substantial”.
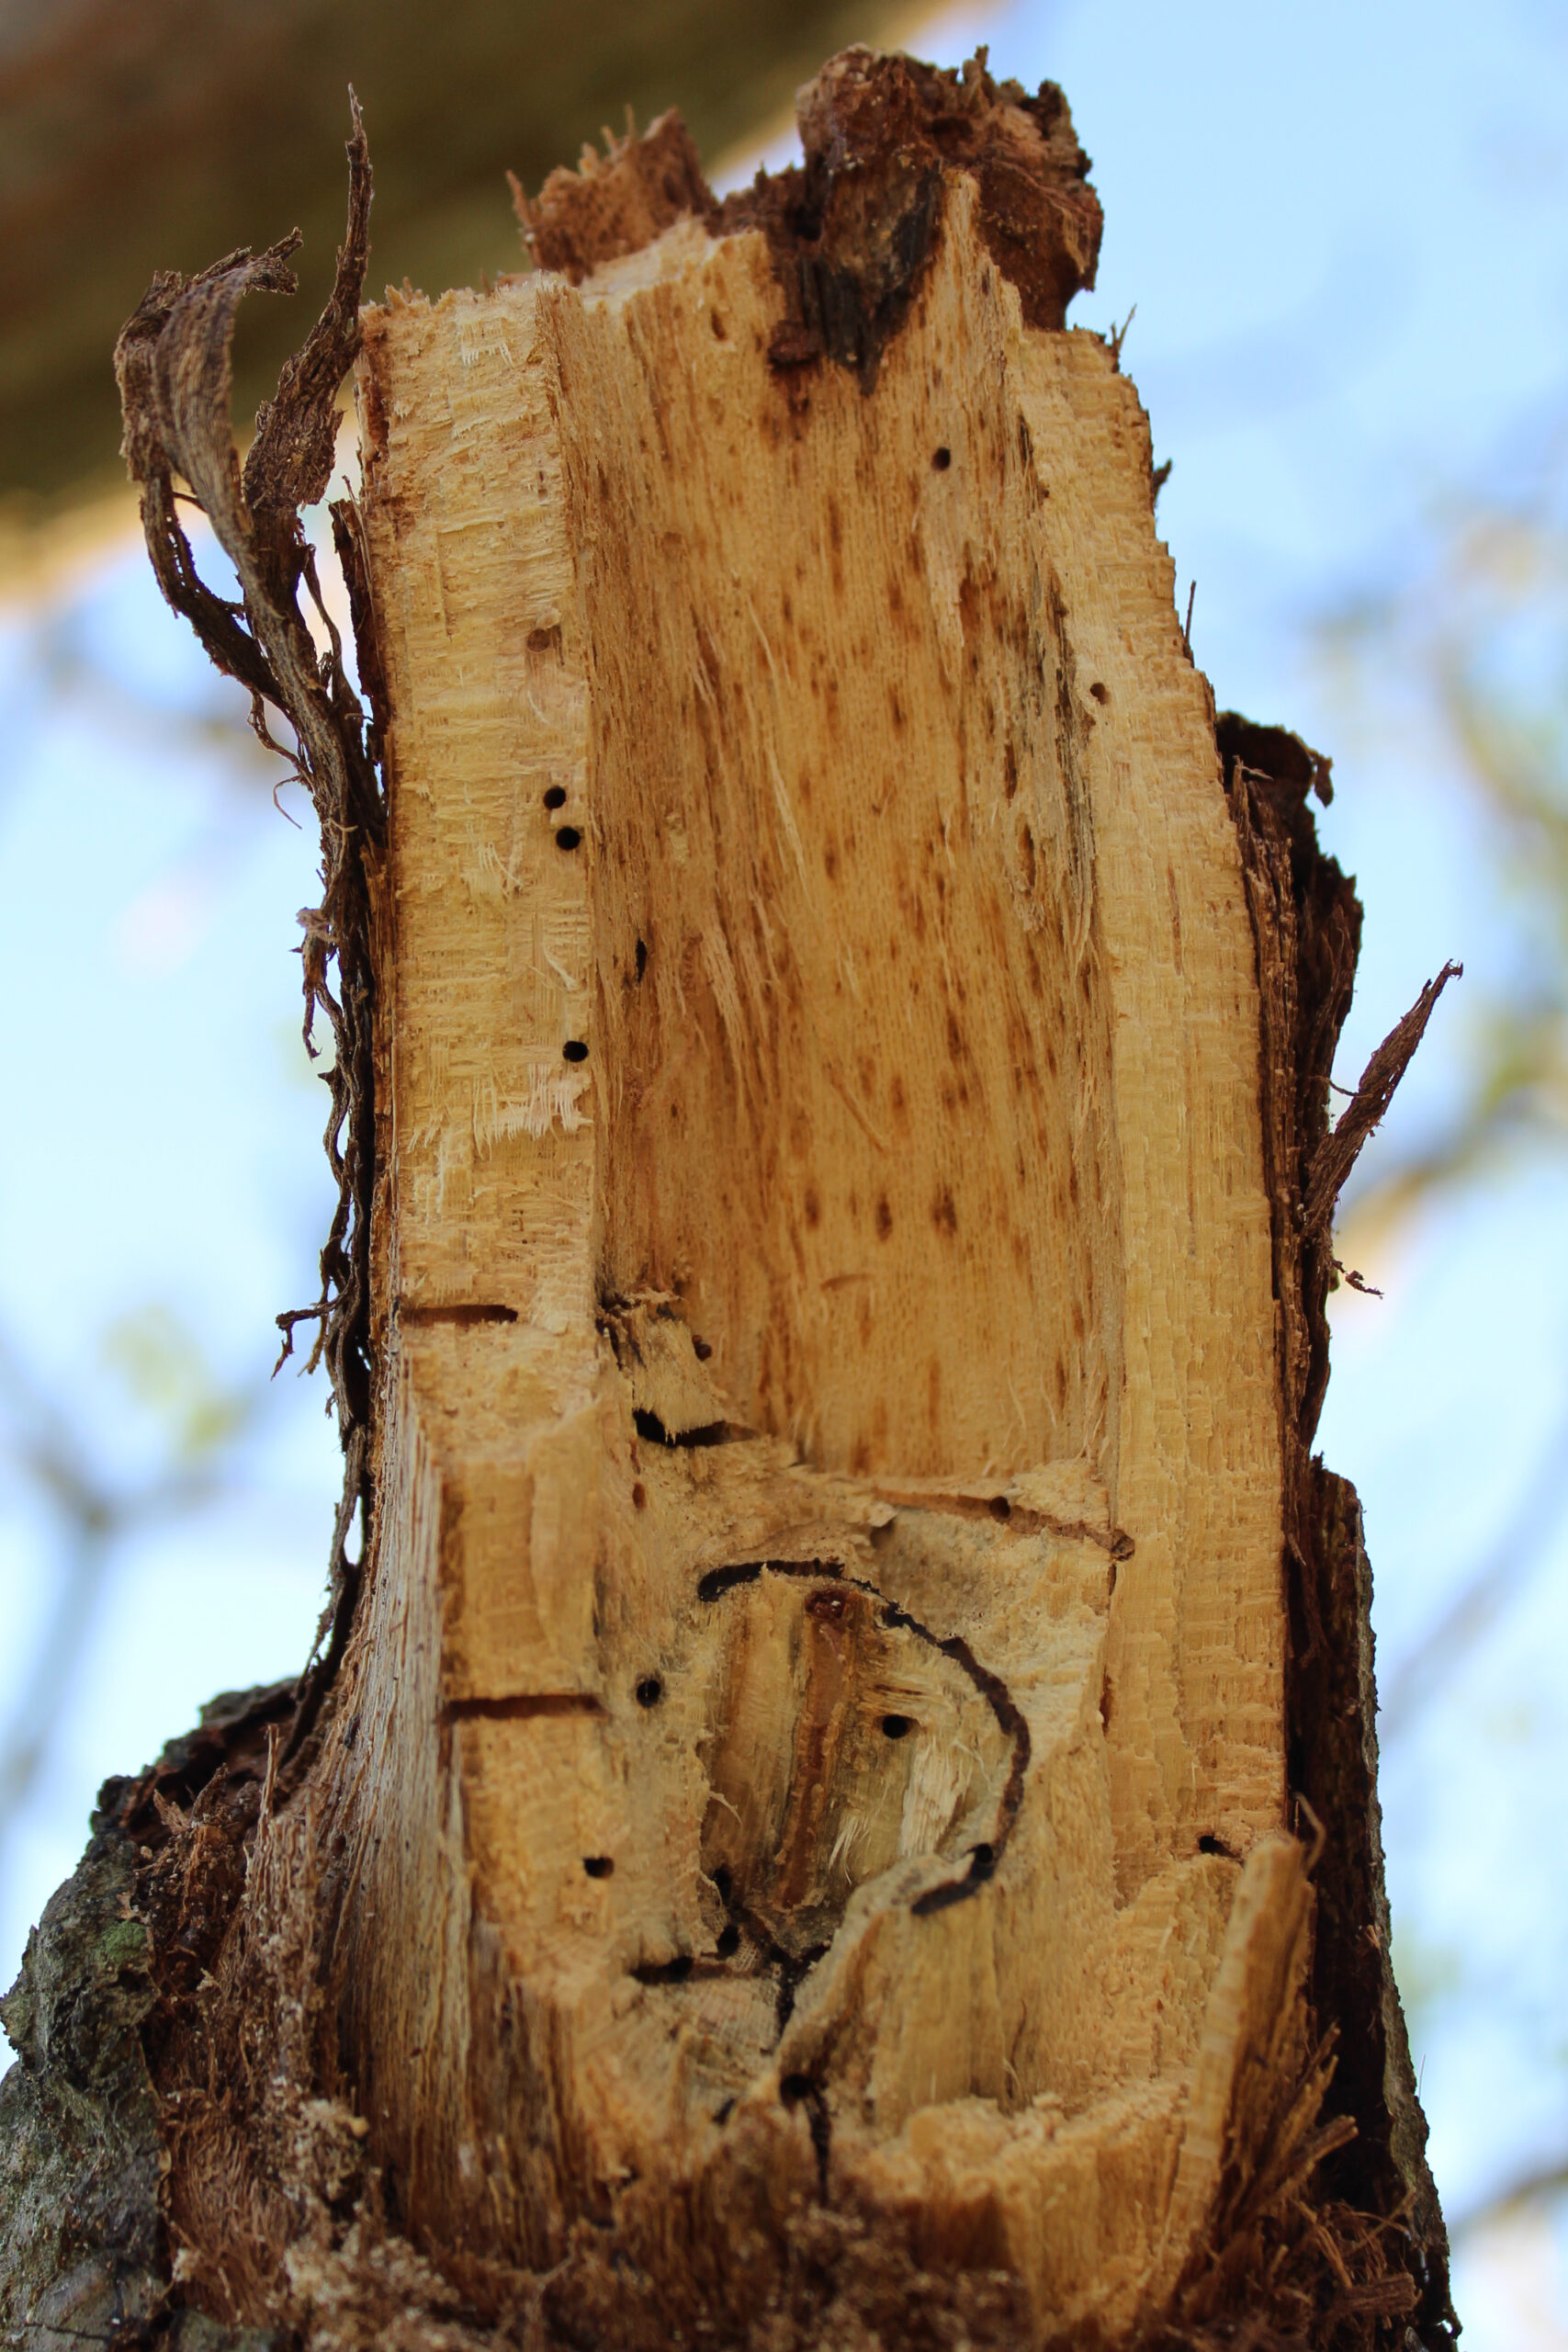
Erythrina caffra in South Africa infested by PSHB; photo by T. Paap

In South America PSHB has spread 3,500 km along the coast since it was detected in Brazil in 2020. While local experts Ceriani Nakamurakare and colleagues (2023) mention attacks on non-indigenous landscaping favorites, Dell, Xu, and Chi (2026) report that in Uruguay a significant number of native species have proved to be reproductive hosts for the beetle.

The PSHB invasion in Western Australia is particularly worrying. The list of hosts has grown rapidly. While 69% are non-native plant species, 8.7% are regionally indigenous and another 21.3% are native to other parts of Australia. Initially authorities attempted to contain the outbreak. They spent $40 million pruning or removing 5,000 trees in the Perth region (Pennisi 2026; unclear whether the figure is in U.S. or Australian dollars). They then decided that eradication was infeasible and shifted the program to management focused on minimizing the risk of further spread. In November 2025, the National Management Group allocated $16.5 million (Australian) to this effort. The state of Western Australia committed $18.8 million for the 2025–26 period, plus $5.1 M for a tree recovery initiative (Dell, Xu, and Chi 2026).

To date, the total budget for PSHB eradication/management from all funding sources has surpassed $92 million. Under the long-term management approach, local governments and communities must assume significant additional expenses for tree removal and replacement (Dell, Xu, and Chi 2026). This team critiqued Australian officials for being slow to engage the public in PSHB detection.

According to the article in Science, the PSHB outbreak has not yet reached the habitats and hosts most likely to support establishment. There, its population could skyrocket (Pennisi 2026).
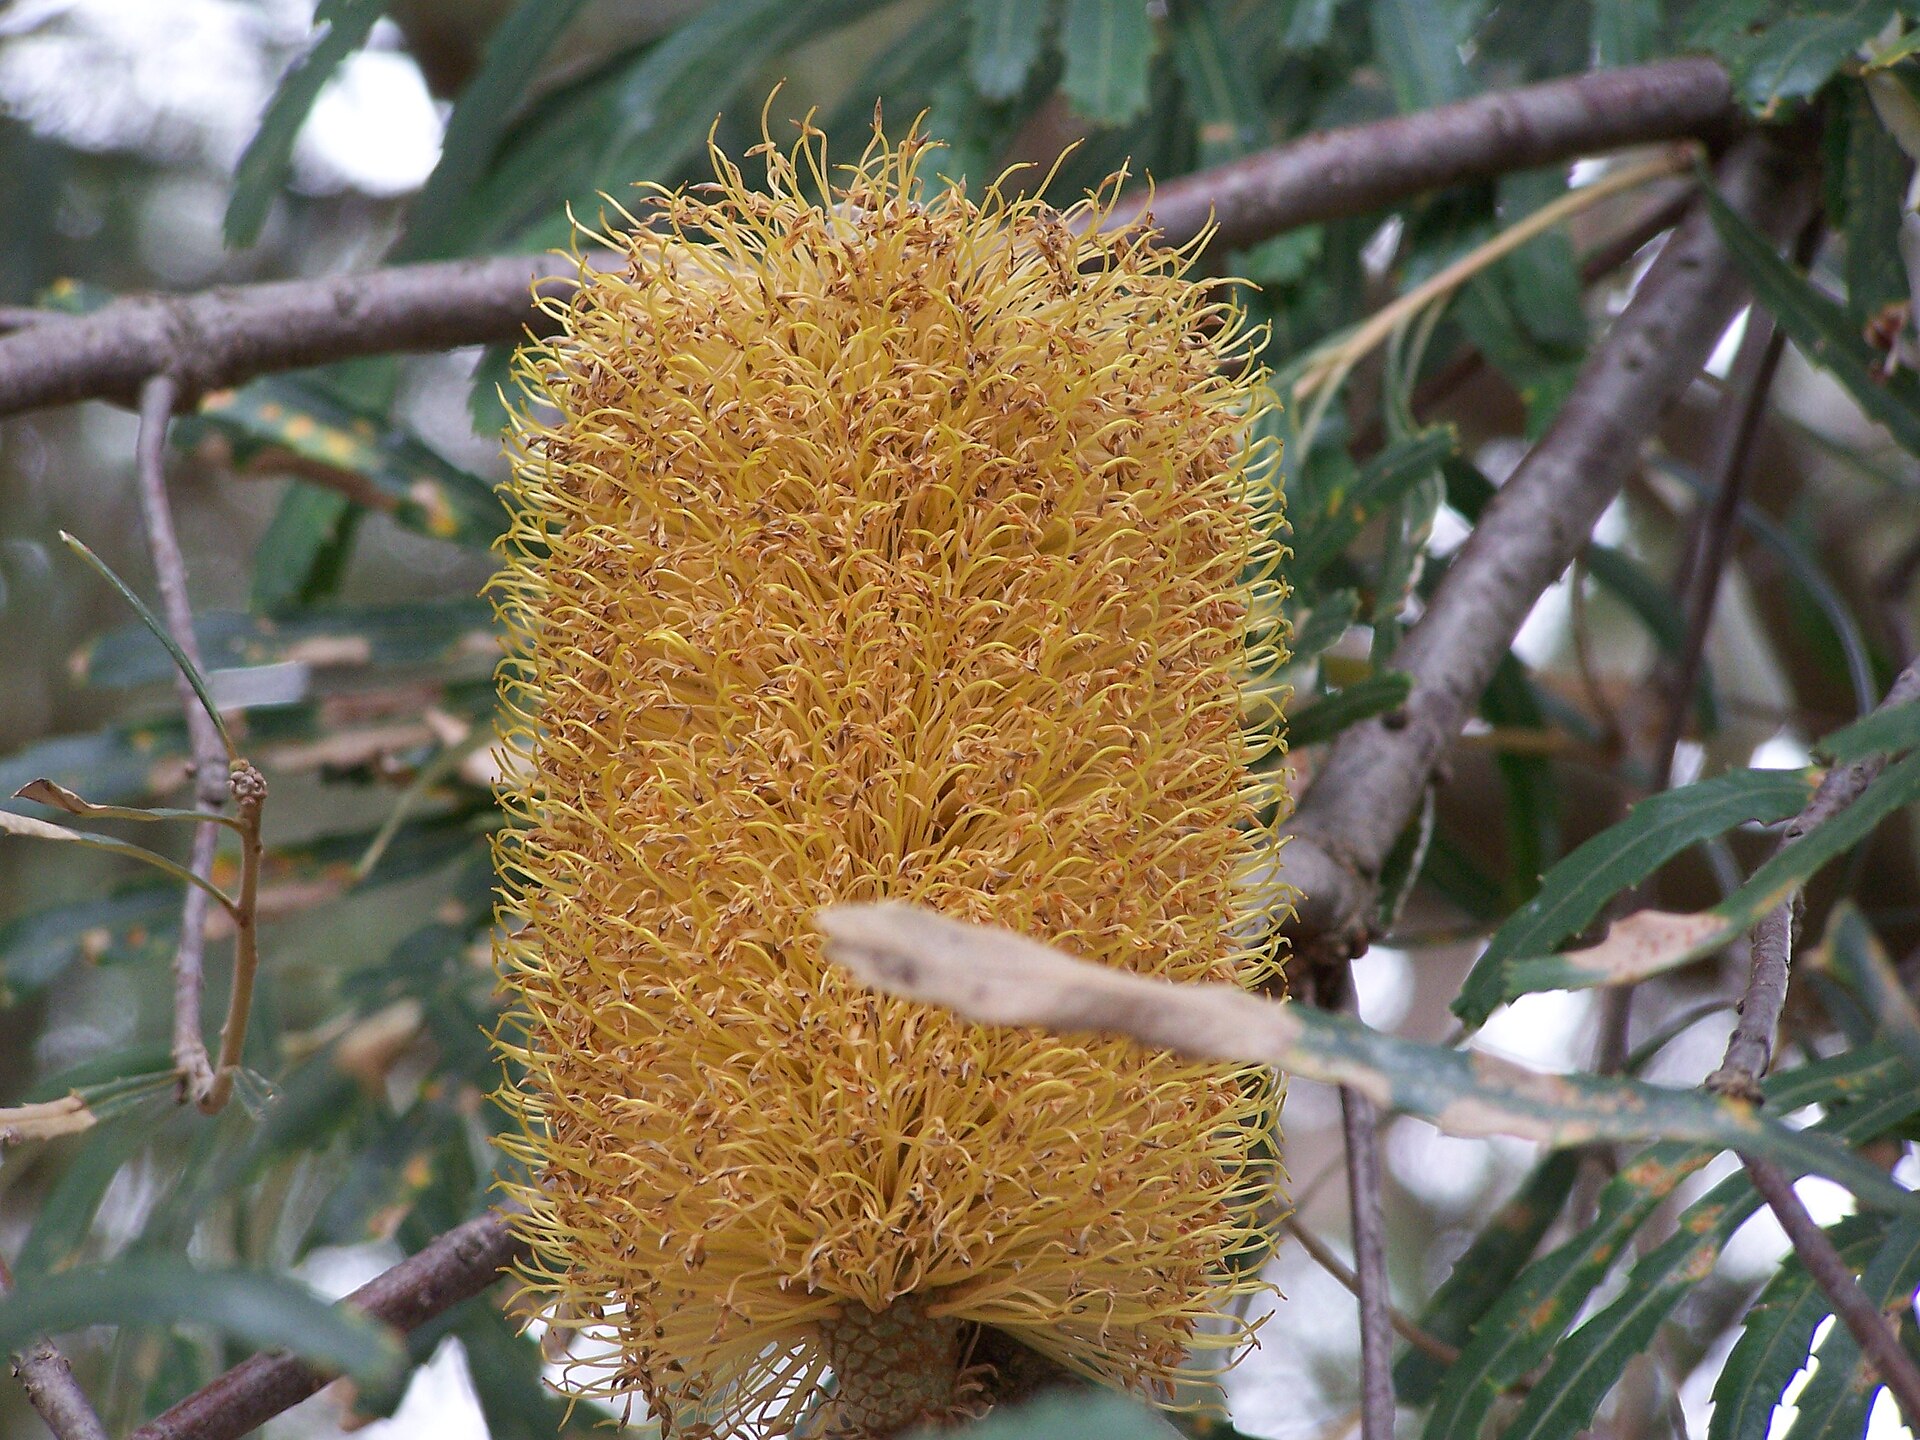
swamp banksia (Bansia littor …) one of the endemic plant species in Western Australia vulnerable to PSHB; photo by Gnagarra via Wikimedia

Upon detection of PSHB in Western Australia, authorities in the state of New South Wales (more than 3,000 km away on the other side of the continent) stepped up surveillance and risk assessment. They determined that 47% of urban trees in Sydney are susceptible to PSHB. Authorities added key PSHB hosts to the list of sentinel trees (i.e., Acer, Cupaniopsis, Ficus, Robinia). The presence of the closely related Euwallacea perbrevis has complicated efforts (Carnegie et al. 2026)

Dell, Xu, and Chi (2026) also describe damage caused by the beetle-fungus complex in Vietnam – that is, in the native range.

Future Damage

Models developed by Lantschner et al. (2026) suggest where populations of E. fornicatus might spread under the rising temperatures and shifting precipitation patterns caused by climate change. The population currently established in southern California could spread into the southeastern U.S., eastern Mexico, and parts of Central America. [I note that many proven host species are either native to or widely planted in southern U.S. states.] Populations in South Africa might spread into the northern part of temperate and subtropical regions of Africa. Beetle populations established in Spain, Israel and Türkiye might spread across the Mediterranean basin. The population in Western Australia could spread to the country’s east – as noted, NSW authorities are already alert to this possibility. Lantschner et al. (2026) raise the caveat that for many of these range expansions to occur the PSHB must cross substantial gaps of unsuitable habitat. Given that their earlier description of how frequently E. fornicatus has exploited human transport to cross oceans, I wonder that they don’t concede that this prerequisite is not likely to be a significant barrier.

Fixing the Problems

Of the references cited here, Pennisi’s article in Science has probably reached the broadest readership. However, it doesn’t discuss how governments and stakeholders can improve the international phytosanitary system. I fear readers will conclude that we are helpless to stop spread of this species or other introductions of similar organisms. The scientific papers offer some steps to improve prevention and detection of ambrosia beetles being transported by trade.

Dell, Xu, and Chi (2026) offer a welcome focus on policy-level changes. I agree with their assertion that real progress depends on more than scientists’ discoveries. They advocate shifting the international phytosanitary system from reactive eradication programs to a more proactive, adaptive, and resilient forest biosecurity systems based on the “One Biosecurity” concept. The proposed new approach will require stronger international collaboration on surveillance, diagnostic protocols, and information sharing; long-term investment in research and surveillance; and improved integration of science, policy, industry, and community. They propose a new framework to facilitate scientists’ engagement with policymakers.

However, in praising South Africa and California for utilizing citizen science and extensive community involvementDell, Xu, and Chi (2026) do not recognize how important individuals have been. In California, John Kabashima led the lobbying campaign to obtain needed government funding. https://www.nivemnic.us/?p=1275

Dell, Xu, and Chi (2026) also address scientists’ criticism of the practice of relying on lists of regulated organisms. This approach allows introduction of lesser-known species with undetermined threat status.

Dell, Xu, and Chi (2026) weigh in on details of surveillance, inspection, regulation, and management responses specific to various settings. For example, noting that only a small proportion of internationally traded wood and wood products is inspected at ports of entry, they advocate tighter phytosanitary certificates (presumably in addition to the ISPM#15 mark) and greater engagement by those in the supply chain. These authors also advocate for more intense inspection of high-risk trade pathways, enhanced surveillance and trapping around ports, and establishment of national pest surveillance programs. They expect emerging technologies e.g., molecular diagnostics, eDNA detection, remote sensing, machine learning, and AI-assisted surveillance to support major improvements in detection and management.

I applaud their attention to the demonstrated inadequacies of ISPM#15 as regards continuing introductions. To see my past advocacy on this topic, scroll down below “Recent Posts”, “Recent Comments” and “Archive” to “Categories and click on “wood packaging”.

Regarding management strategies, they describe challenges hindering use of chemical attractants and treatments, use of entomopathogenic fungi as biological control agents, and breeding trees resistant to the beetle-fungus complex. Nevertheless, they consider it essential to preserve the genetics of endangered species.

Dell, Xu, and Chi (2026) also review gaps in scientific understanding of ambrosia beetles, their host interaction and fungal symbionts. Closing these gaps is essential for developing more effective long-term management strategies. They assert that the substantial increase in funding needed to do this work is warranted given the level of damage caused by the PSHB and other ambrosia beetles.

Lantschner et al. (2026) tie their recommendations to ambrosia beetles specifically. They say that the different invasion patterns of E. fornicatus and E. perbrevis demonstrate that surveillance and management tactics must be species-specific. (This necessity adds to the complexity and resource demands of the task.) They also urge study of the PSHB’s broader microbiome, which influences beetle fitness, symbiosis stability, and invasion success. Research should also explore the extent to which environmental stressors, e.g., drought, temperature extremes, and mechanical damage, influence PSHB attacks across different environments; and whether semiochemicals have any role in insect behavior.

Finally, Lantschner et al. (2026) warn that species’ occurrence data based solely on climatic factors might not accurately reflect its possible range. This is because both biotic interactions and land-use patterns play a role in determining where a pest is present.

SOURCES

Bierman, A., F. Roets, J.S. Terblanche. 2022. Pop structure of the invasive ambrosia beetle, Euwallacea fornicatus, indicates multiple intros into South Africa. Biol Invasions (2022) 24:2301–2312 https://doi.org/10.1007/s10530-022-02801-x

Carnegie AJ, Summerell BA, Trollip C, Tovar F, Smith DI and McDonald J (2026) Sentinel trees for early detection of non-native forest pests and pathogens in AU.

Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Ceriani-Nakamurakare, E. A.J. Johnson and D.F. Gomez. 2023. Uncharted Territories: First Report of Euwallacea fornicatus (Eichoff) in South America with new reproductive hosts records. Zootaxa, 5325 (2), 289-297. https://doi.org/10.11646/zootaxa.f325.2.10

Dell, B., W. Xu, and N.M. Chi. 2026. Polyphagous Shot Hole Borer, a Global Threat to Forest Plantations, Green Infrastructure, and Biodiversity: Status, Challenges, and Solutions. Forests 2026, 17, 832

Lantschner, M.V., E. Ceriani-Nakamurakare, A.J. Johnson, A.I. Cognato, S.M. Smith, D.F. Gomez. 2026. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis (Coleoptera: Scolytinae), two global emerging pests. J Pest Sci 99, 100 (2026). https://doi.org/10.1007/s10340-026-02070-w

Pennisi, E. 2026. Tree-killing beetle is spreading to urban forests around the world. As researchers piece together the pest’s global trek, countries are working to contain the growing threat. Science 15 July 2026

Rabaglia, R.J., S.A. Dole, and A.I. Cognato. 2006. Review of American Xyleborina (Coleoptera: Curculionidae: Scolytinae) Occurring North of Mexico, with an Illustrated Key. Ann. Entomol. Soc. Am. 99: 1034–1056.

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org


U.S. imports continue growing … as does risk of introductions

As I have documented in the past, wood packaging (crates, pallets, spools for cable, etc.) remains a pathway for introduction of tree-killing insects, including those that vector pathogens. Visit previous blogs describing continuing failures of the international standard by scrolling below “Comments” and “Archive” to “Categories” and click on “wood packaging”.

Because of the associated risk, I report on volumes of incoming trade containers, called “TEUs”. This acronym stands for “twenty-foot equivalent”. I focus on expanding import volumes from Asia into East and Gulf Coast ports because 1) ecological similarities between East Asia and eastern North America facilitate establishment of species from Asia into this region; 2) China has a particularly poor record of non-compliance with the international standard; 3) U.S. phytosanitary officials at eastern ports might be less prepared to handle the volume.

So what is the situation in Autumn 2026?

U.S. imports have been rising – despite tariffs, trade wars, shooting wars, and weather challenges. The following information comes from articles posted by the Journal of Commerce. Unfortunately, JOC articles are behind a paywall.

In 2025, the top nine U.S. ports handled 49.5 M total TEUs, loaded and empty, the third highest number after 2022 and 2021. People in trade expect the overall U.S. container trade to grow between 2 and 3% annually. A 3% growth rate would put total U.S. container handling (imports and exports) at just over 66 million TEUs by 2035 (Michael Angell, Oct 20, 2026).

Higher import volumes are linked to the data center construction boom (Mark Szakonyi, October 2, 2026). For example, the Port of Houston saw a 41% increase in imports of wiring, electrical transformers and switches, refrigeration equipment, and lithium-ion batteries – to 80,953 TEUs (Michael Angell, October 5, 2026).

U.S. east coast ports saw a 28% increase in volumes from Southeast Asia over the past two years (Michael Angell, Oct 20, 2026). In recent months, however, U.S. importers have shifted sourcing back to China because of easing U.S. tariffs and lower energy costs than in Southeast Asia (Mark Szakonyi, October 2, 2026.

The ports of Los Angeles and Long Beach have been handling record or near-record container volumes over the past four months as retailers responded to changing tariff deadlines and supply chain challenges caused by congestion at Chinese ports and drought-caused draft limitations at the Panama Canal (Bill Mongelluzzo, October 30, 2026).

Supply chain challenges in addition to the shallow water in the Panama Canal (which has restricted ship passages) include 13 typhoons in East Asia, some of which have forced closure of export harbors in China, Taiwan, and possibly Japan (Keith Wallis, October 23, 2026). This month devastating floods in the Four Corners area have completely disrupts rail transport from the California ports to the Midwest and East (Bill Mongelluzzo, October 27, 2026).

A looming complication is the possible strike by security personnel at Los Angeles and Long Beach (Bill Mongelluzzo, October 30, 2026; Ari Ashe, October 27, 2026).

Port of Houston

Imports from Asia to East and Gulf Coast Ports Continue to Rise

Houston saw the largest increase percentage-wise of major U.S. ports from Asia — up 11.7% from the same eight-month period (through August) in 2025. This year, 792,419 TEUs from Asia have entered Houston. (As noted above, 10% of these containers held equipment for data centers). Overall, through this period, Houston received 5% more loaded import TEUs (1.4 million) than over the same period a year ago. Other ports also received higher numbers of containers from Asia, although significantly lower percentages: Savannah imports rose by 4.5%; Los Angeles by 4%; and New York-New Jersey by 3.2%. Not all ports saw gains: Seattle/Tacoma received 14% fewer containers from Asia, Charleston 6.4% fewer, Oakland 3% fewer (Michael Angell, October 5, 2026).

Expansions Continue at East and Gulf Coast Ports

See earlier reports on these expansions by scrolling below “Comments” and “Archive” to “Categories” and click on “wood packaging”.

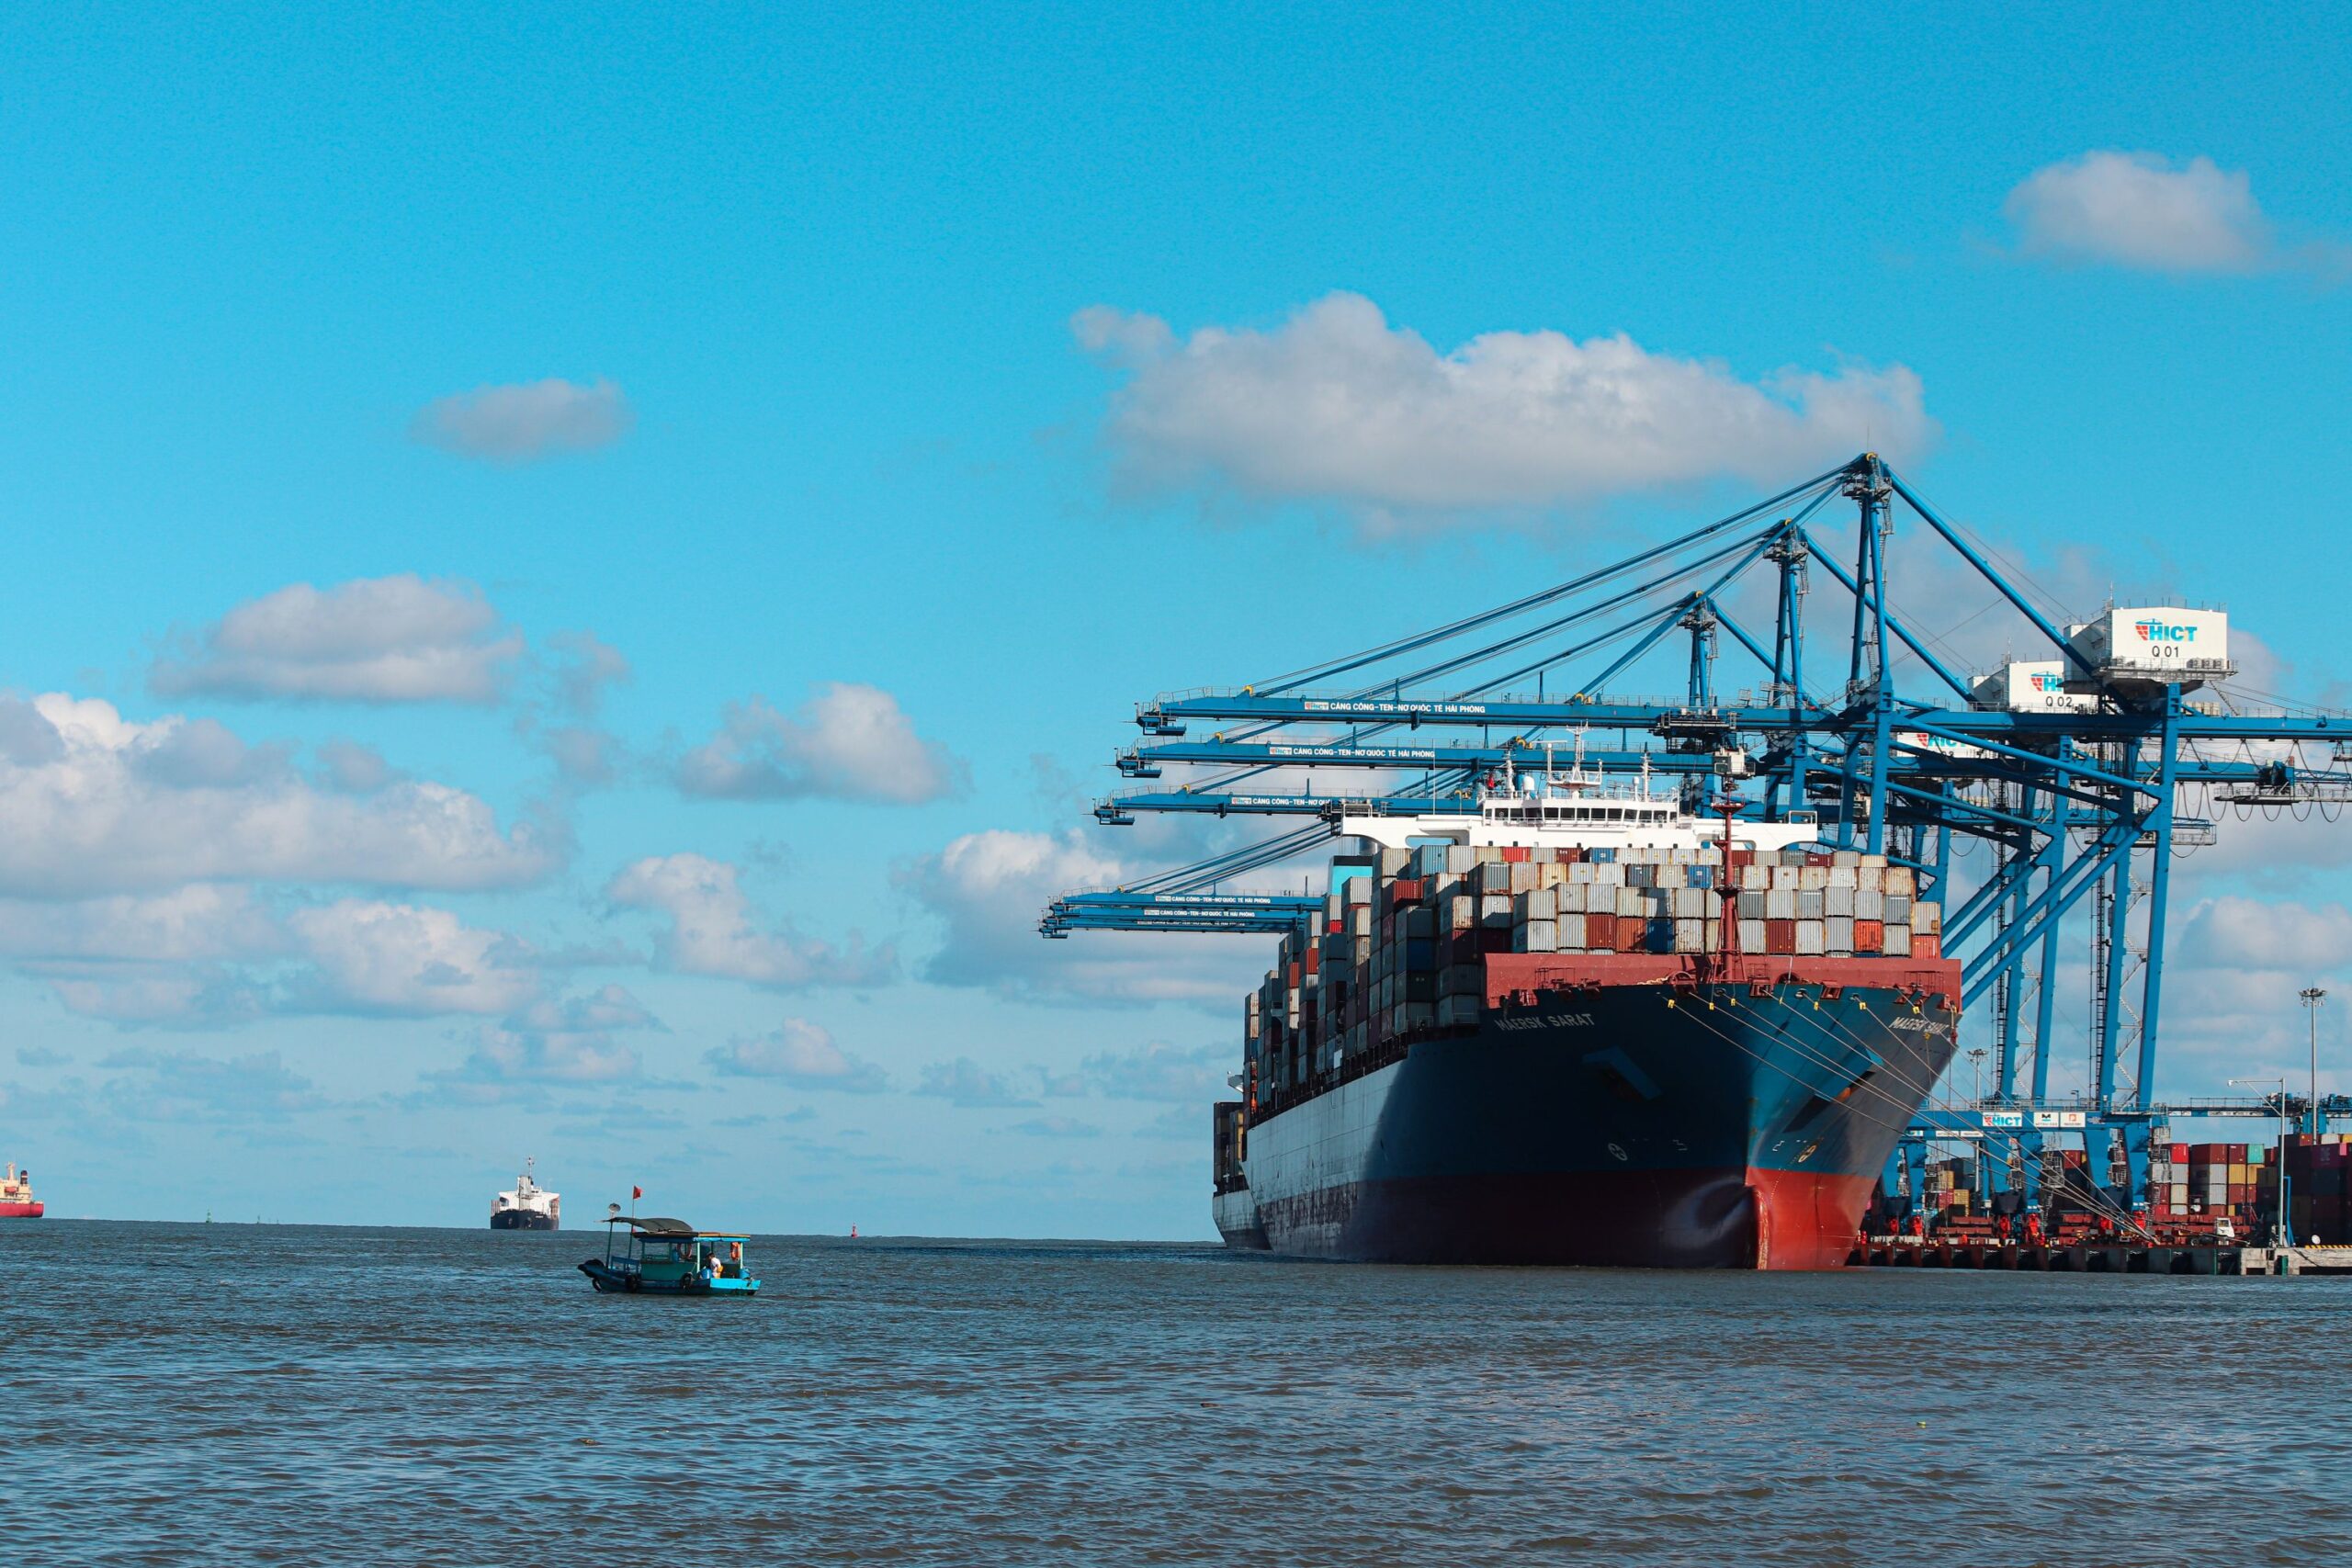
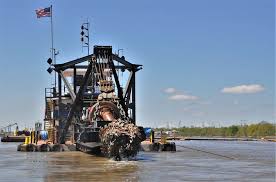
Container ports along the U.S. East and Gulf are in the process of or planning major expansions through the 2030s in anticipation of increasing volumes from places other than China. Projects include expanding the ports’ rail networks to reach inland markets now served mostly by the West Coast. Three projects will ramp up capacity to gradually to 6.8 million TEUs by completion a decade from now. Baltimore and Wilmington, Delaware broke ground earlier this year on their expansions. Savannah has obtained needed permits for constructing a third terminal. It also will build a new container yard. A fourth project at Norfolk will eventually add another 3.4 M TEUs to East Coast capacity. Farther in the future, Philadelphia has obtained funding to double its capacity, which would add another one million TEUs (Michael Angell, October 20, 2026). Savannah was the port of introduction of the redbay ambrosia beetle and its associated fungus as well as two conspicuous arthropods that are not forest pests, the East Asian Joro spider and yellow-legged hornet. Charleston might have been one of many ports of introduction of the Asian longhorned beetle.

dredging the Port of Savannah

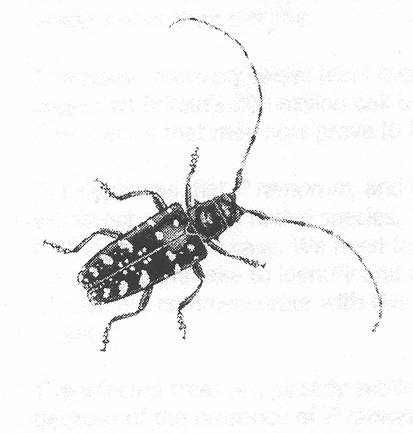
Some ports have found a different, probably cheaper, way to increase capacity. The Port of New York-New Jersey is upgrading equipment so it can stack containers up to six high, thus storing a third more containers in the same space as currently. This adjustment could add another 1.5 M TEUs to the port’s current capacity of ~10 M TEUs (Michael Angell, October 20, 2026). The New York metropolitan area has been the site of numerous pest introductions, most notably the original establishment of the Asian longhorned beetle.

Asian longhorned beetle

Gulf Coast ports are also expanding. New Orleans has awarded preliminary contracts for building the Louisiana International Terminal. Houston is fast-tracking a permit for a third container terminal. These projects could add ~6.3 M TEUs in new container handling capacity on the Gulf Coast through the 2030s. More is planned. Corpus Christi has signed a lease to build its first container terminal and Mobile is dredging its harbor. These projects would raise the Gulf Coast container handling capacity to 7 million TEUs (Michael Angell, October 20, 2026).

Port expansion is not limited to the United States. The port of St. John, New Brunswick, announced it will receive C$463 million (US$330 million) from federal and provincial governments and the private sector to increase container handling capacity from 850,000 TEU to one million TEUs. The project includes dredging to allow deeper-draft ships to call more frequently, expanding port warehouses, building a new customs inspection facility, and improvements to the port’s rail infrastructure. Import volumes are growing: the 239,364 TEUs handled in 2025 was a 29% increase over 2024. Port St. John already can handle super-post Panamax ships with a 56-foot draft. (Michael Angell, October 22, 2026). Halifax was the port of introduction of three tree-killing pests: beech bark disease in the 1890s; brown spruce longhorned beetle in 1999; and beech leaf-mining weevil in 2012.

symptoms of beech bark disease; photo courtesy of Bugwood

Labor unions at Halifax and Montreal have recently signed agreements that make strikes unlikely (Journal of Commerce staff | October 23, 2026).

UPDATE

US imports from Asia in October jumped to 1.9 million TEUs — an all-time high for any month.

The ports of Los Angeles and Long Beach have handled the highest cargo volumes in their history. Port officials expect the complex to handle 268,000 incoming TEUs during the week of November 16th. That number will increase to 315,000 next week before dipping to 289,000 laden TEUs for the week of Nov. 22-28. The typical import total is about 200,000 laden TEUs per week (Bill Mongelluzzo, November 16, 2026).

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Rapid growth of a coalition tackling invasive plants in Virginia!

The Virginia Invasive Plants Coalition was formed at December 2023. Seventy-six organizations participated in the formative meeting. The Coalition now boasts 113 members. CISP joined the coalition this autumn.

The Coalition’s purpose of is to identify and carry forward statewide efforts to make dramatic progress against invasive plants support the use of native plants. Members work collectively on ten initiatives:

  • awareness & education;
  • resource development;
  • support & implement a Virginia Invasive Species Management Plan;
  • create or provide expertise, incentives, and access to funds to help private land stewards mitigate invasive species
  • limit access to invasive plant;
  • research to identify & address knowledge gaps;
  • remove invasive plants & restore with native plants;
  • ensure equitable access;
  • build collaborative networks;
  • ensure that Virginia adopts policies that support reduction of invasive plants & reverse the damage they cause

I rejoice that the Coalition explicitly includes advocacy for state-level policy. I wonder whether – over time – VIPC members might consider advocating for more effective federal policies.

I also wonder whether organizations concerned about invasive species have formed similar broad and action-oriented coalitions in other states.

I will focus here on two VIPC efforts.

Virginia State Capitol; photo by Tony Fischer via Flickr
  1. Policy

Virginia currently has two lists of invasive plants. The Department of Agriculture and Consumer Services (VDACS) lists “noxious weeds”. It currently contains 26 species in three tiers. It is illegal to sell species on this list. The Department of Conservation and Recreation (DCR) maintains the Virginia invasive plant list. The list contains 103 species. It includes a list of species identified to spur “early detection”. All noxious weeds are also included on the “invasive” list, but not all “invasive” plants are listed as noxious weeds.

burning bush – on the DCR invasive plant list but not the VDACS noxious weed list; photo by F.T. Campbell in Fairfax County, Virginia

VIPC is a member of the Virginia Conservation Network. This coalition has developed a conservation agenda for 2027; the agenda has four categories: water; land & wildlife conservation; climate & energy; land use & transportation. “Preventing harm from invasive plants” is included under the “Native habitats & species” chapter.

In 2026 the state legislature adopted four laws that:

a) added invasive plant management to the powers of service districts; [A “service district” is a defined geographic area within a local government established to provide additional, more complete, or more timely governmental services than those generally provided to the rest of the locality];

b) removed the “commercial viability” loophole from the state’s noxious weeds law;

c) required Virginia’s Department of Transportation to create a plan for managing invasive plants along  public roadways; &

d) allowed volunteers to use herbicides on state-owned public lands when under supervision of a licensed commercial pesticide applicator.

Legislation also now requires retail outlets to place warning signs near each invasive plant species offered for sale (effective January 2027); partially funds the Virginia Invasive Species Management Plan; prohibits state agencies from planting, selling, or propagating invasive plants; requires tradespersons to provide written notification to property owners for all plants proposed for installation that are included on the list of invasive plants; & allows localities to permit the supervised use of herbicides by volunteers on public lands.

The Virginia Conservation Network considers these actions to be too limited. The VIPC asks its member organizations to advocate for

  • Require property sellers to disclose the presence of Japanese knotweed (Reynoutria / Fallopia japonica or Polygonum cuspidatum) on a property they are selling because it can disrupt underground infrastructure.
  • Tightening label language regarding whether a plant is “sterile”.
  • Require those clearing property for development to plant cover crops to forestall weed invasions if there is a delay in further work.
Japanese knotweed; photo by Will Parson, Chesapeake Bay Foundation

Perhaps in future the Network might broaden members’ concern about the loss of forest canopies to include insects and pathogens that kill trees?

2) Surveying nurseries to find those selling invasive plant species.

VIPC members carried out surveys in 2025 and again in 2026. The 2026 surveyors visited 122 nurseries in 60 locations across the Commonwealth. This was 42% more retailers than the 2025 survey. One-third of the nursery locations were in the Northern Virginia suburbs of Washington, D.C.

butterfly bush Buddleya davidii; photo from Free Public Images

The 2026 surveyors found a 23% decrease in invasive plant species being offered per retailer. Twelve percent of the garden centers had no invasive species for sale. This was more than triple the number found during 2025. However, one garden center was selling 24 of the 39 invasive plant species. The most commonly detected invasive species are:

  • butterfly bush — found during 95 visits; [see Douglas Tallamy on why butterfly larvae cannot use this plant.]
  • species found during 58 to 79 visits were nandina, English ivy, periwinkle, moneywort, and Japanese barberry;
  • Japanese spirea and burning bush were found during 45 or 44 visits;
  • Two ornamental grasses, Chinese silvergrass and fountain grass, were found during 30 or 29 visits;
  • species found during 19 to 16 visits were greater periwinkle, leatherleaf mahonia, Chinese privet, and winter creeper;
  • species found during eleven to eight visits were Chinese wisteria, mimosa, water hyacinth, yellow flag, sweet autumn clematis, and border privet;
  • species found during five or four visits were creeping Charlie, Callery pear, golden bamboo, and Norway maple.

Invasive species found at a smaller percentage of Virginia garden centers in 2026 than in 2025 were butterfly bush, nandina, English ivy, periwinkle, greater periwinkle, Chinese privet, winter creeper, sweet autumn clematis, border privet, Callery pear, and linden arrowwood.

Invasive species found at a higher percentage of retailers in 2026 than in 2025 were moneywort, Japanese spirea, Chinese silvergrass, mimosa, water hyacinth, yellow flag, and Japanese honeysuckle (Lonicera japonica). The last species is on the Virginia Noxious Weeds List, so sale is illegal.

Invasive species found at the same percentage of Virginia garden centers in 2026 as in 2025 were Japanese barberry, burning bush, fountain grass, leatherleaf mahonia, Chinese wisteria, creeping Charlie, golden bamboo, Norway maple, five-leaf akebia, parrotfeather beefsteak plant, Italian arum, white mulberry, Chinese tallow-tree, and trifoliate orange.

Invasive species not found offered for sale by surveyed garden centers in 2026 were Amur honeysuckle*, Autumn olive*, Brazilian waterweed, cinnamon vine, cogon grass*, crown-vetch, incised fumewort*, marsh dewflower, Morrow’s honeysuckle, Oriental bittersweet*, porcelain-berry*, purple loosestrife, ravenna grass, royal paulownia, shrubby bushclover*, Siberian elm, tartarian honeysuckle, thorny olive, tree-of-heaven*, wineberry, and winter honeysuckle. (*indicates plants listed on the Virginia Noxious Weeds List.)

oriental bittersweet; on Virginia’s noxious weed list (tier 3); Picture This

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Invasive species’ spread facilitated by inconsistent approaches

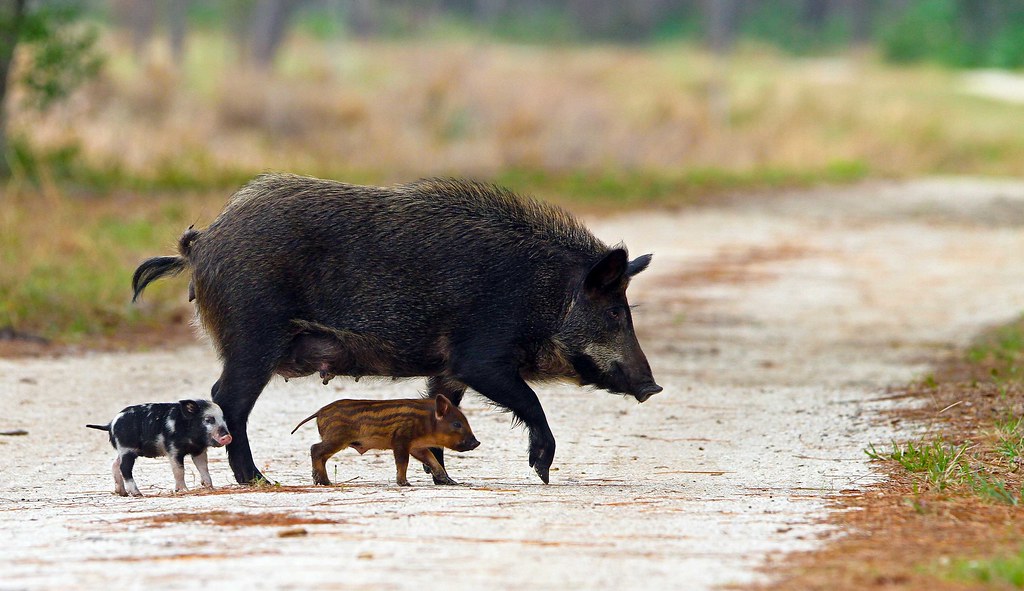
feral hogs — one the invasive species on which state approaches vary; photo by Creg Oneal via Flickr

Several groups of scientists are addressing systemic problems that impede efforts to counter bioinvasions. One of those problems is the lack of a consistent approach in federal systems. 

Drake et al. (2026) (full citation at the end of this blog) evaluate the impacts of this situation in the United States where – they argue – the national government has been slow to adopt overarching policies and provide adequate and dependable funds to implement them. The result is a patchwork of varying – even clashing – regulations and differing levels of effort that undermine program efficacy. Conflicting approaches add to such well-known challenges as limited budgets and evolving goals. They recommend applying such existing frameworks as the National Invasive Species Council’s (NISC) Early Detection / Rapid Response framework or One Biosecurity to facilitate integration and cooperation among the large variety of sectors affected. (NISC’s purpose is to coordinate federal agencies’ programs. The Council has no official role vis a vis state programs. Still, there is no legal impediment to states adopting any NISC approach which they consider appropriate.) At the same time Drake et al. (2026) warn against imposing too great uniformity or lacking flexibility.

I regret that Drake et al. (2026) do not mention the National Plant Board. The NPB focuses on managing plant pests (insects, pathogens, etc.) and invasive plants. The NPB recently celebrated its centennial anniversary. States have created fora under the NPB in which they exchange experiences with the goal of coordinating their efforts.

With respect to animal invaders (other than plant pests) or disease or parasite threats to animals, I believe there is no equivalent to the NPB. The Association of State Wildlife Agencies (AFWA) has an invasive species committee which discusses issues of general concern (see agenda from one of its meetings here).  This effort is much more recent than the NPB. It is similar in that it is consultative, with no authority to enforce a common approach.

Findings

Drake et al. (2026) explore the extent to which American states apply similar vs. different approaches to managing invasive species as a group and plants, invertebrates, and vertebrates separately. Lack of data forced them to exclude fungi and other microorganisms. They focused on 21 contiguous states in the eastern part of the country. They also compared the states’ lists of regulated species to national lists of invasive species compiled by the United States’ Register of Invasive and Introduced Species (US-RIIS) (Simpson et al., 2022; Simpson and Eyler, 2018) and U.S. Geological Survey Non-indigenous Aquatic Species database (NAS; U.S. Geological Survey, 2023).

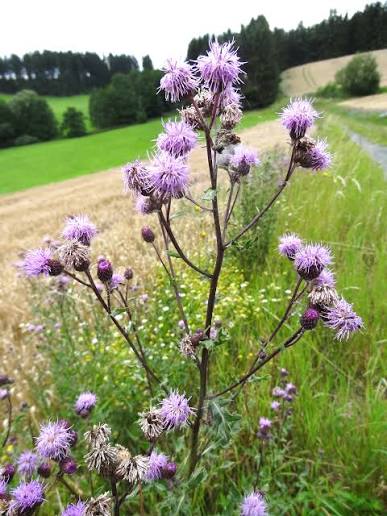
A literature search revealed 1,117 state statutes, regulations, and similar policy documents that pertain to invasive species. One third of these documents (n = 448) named at least one taxon at the genus or species level. Of these, 35.3% named one or more plant species; 19.9% named one or more invertebrate; and 44.8% named vertebrates. Overall, 60.5% of these species were listed by only one state. Viewed by taxonomic group, this broke down to 40.6% of plant species, 60.6% of invertebrates, and 56.4% of vertebrates. Only four species are regulated in all 21 states = western (European) honeybee (Apis mellifera); and three agricultural weeds, creeping thistle (Cirsium arvense), quackgrass (Elymus repens), and dodder (Cuscuta species).

Cirsium arvense; photo by USchmidt via WikiMedia

Drake et al. (2026) found neighboring states did not share similar species lists or approaches. Consistency was even less at the regional scale, particularly when managing invasive invertebrates or vertebrates. The absence of a unified approach means that proactive states are susceptible to invasion from neighboring states which take a less vigorous stance. Since managing invasive species becomes more difficult and costly as the invasion progresses, undermining proactive policies undercuts efficiency.

Even when the national government does act, it lacks a unified approach. No federal legislation mandates a central authority to direct and implement IAS detection and response. The National Invasive Species Council (NISC), established by Executive Order 13112 in 1999, is supposed to provide high-level leadership to help overcome barriers to communication and promote collaboration among the several federal agencies bearing responsibility for various aspects of the issue. Authors, e.g., Reaser, Simpson, et al. (2020); Simberloff et al. (2020), say NISC’s effectiveness has been undermined by inconsistent funding and vacillating political support from policy-level leaders.

Drake et al. (2026) also assessed which of the 21 states took action proactively. Two plant species were listed by name by all 21 states: quackgrass (Elymus repens) and creeping thistle (Cirsium arvense). They called three states (14.3%) “pro-active” because they regulated quackgrass before it was detected in the state. Four states (19%) did the same regarding creeping thistle. The one invertebrate species listed by all 21 states, the western (European) honeybee, was established in these states before they began addressing invasive species, so it is not a test of states’ forethought.  

Of course, the policy goals differ between the two plant species and the honeybee: the former are considered damaging so policies focus on their control and management, whereas the honeybee is valued for pollination and honey production so policies aim at protecting it. There is no federal legislation regulating Apis mellifera individuals already in the country. State regulations governing interstate movement are the usual jumble of approaches. Drake et al. (2026) says this lack of consistency can increase the risk that introduced pathogens, pests, and undesirable subspecies (i.e., “Africanized” bees) will spread. They note that this chaos reigns despite bees’ importance to the agricultural sector.

Florida had policies governing the most species (345), Vermont the least (67). More surprising to me, New York regulated the most plant species (161); Mississippi the most invertebrates (105), and Virginia the most vertebrates (189).

Collectively the states regulate three times more species than appear on either national registry: 1,862 species in the state database versus 630 in US-RIIS or NAS databases. The states regulated a proportionally larger number of plant species and much smaller proportion of vertebrates. The number of species named in both state and federal databases were 360 plant species (57.1%), 170 invertebrates (28.4%), and 91 vertebrates (14.4%). The difference between federal and state lists is further magnified by the fact that significant numbers of species listed on the federal databases are managed by only one state: 143 plant species (48.3%), 86 invertebrates (29.1%), and 28 vertebrates (9.5%). In other words, only 217 plant species, 84 invertebrate species, and 63 of vertebrate species designated as invasive by federal databases were being managed by more than one state.

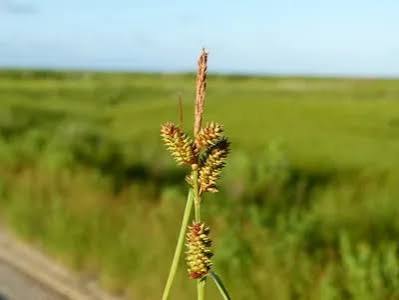
Carex extensa – one of plant species listed as invasive by USGS but not regulated by any of the 21 states; photo by botanygirl via Picture This

The survey identified a wide range of state agencies that have at least some responsibility for managing invasive species. These agencies’ principal concerns are agricultural, plant, or livestock industries; wildlife, fisheries, and recreation; forestry, mining, and natural resources; marine resources; public and environmental health; transportation, utilities, and commerce; and administration, education, specific locations, and all other types. Agriculture agencies are overwhelmingly responsible for invasive plants, insects, and arthropods; and almost equal to Fish and Wildlife departments in the case of managing molluscs. F&W departments are most often responsible for mammals, fish, crustaceans, amphibians and reptiles. Public and environmental health agencies are a distant second as regards responsibility for plants and arthropods, and third re: insects. Administration/education/specific location agencies are third most frequently given responsibility for plants; they hardly appear for other categories. Transport and commerce ranked fourth (nearly the same as public health agencies) for managing insects.

More than half of state policy measures (55.4%) related to terrestrial species, habitats, and pathways; 17.1% related to aquatic species, habitat, and introduction pathways; and 27.5% related to both.

Considering all species named in each state’s policy codes, about half of the listed taxa in each focal state’s policies are also listed by at least one neighboring state. At the regional level, overlapping or consistent policies declined to about 19% of the species. It doesn’t surprise me that New England states rank high in cooperation. Nor that the least number of species also regulated by neighboring states applies to Florida; the “sunshine state” is semitropical and has many types of ecosystems probably not present in Alabama or Georgia.

Once again, consistency is higher for plant species than the animal taxa. Among-neighbor overlap for plant taxa is ~69-70%, for invertebrates is ~50%, and for vertebrates only about a third. At the regional level, overlap is ~28% for plant species, ~18% for invertebrates, and 14% or less for vertebrates.

Drake et al. (2026) present case studies on several species to illustrate the breadth and depth of policy inconsistency, coordination, and implementation. The species studied are three of the four species regulated by all 21 states in the database; and three others selected to be emblematic of plant, invertebrate, and vertebrate taxonomic groups. The representative species for invertebrates is the emerald ash borer (EAB; Agrilus planipennis); the illustrative species for vertebrates is feral pigs (Sus scrofa). 

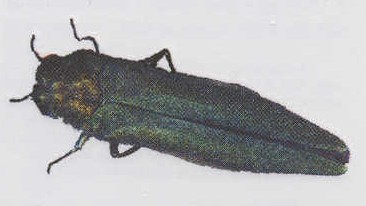
Drake et al. (2026) report that the EAB had been detected in all but two of the 21 states in their study – Florida and Mississippi (EAB has now been detected in the state). There was a federal quarantine until early 2021. Still, only 10 states (47.6%) have a policy regulating EAB per se. Nine states had acted proactively; this was the highest proportion among all the species analyzed, probably because the beetle spread so quickly and had such obvious and severe impacts observed.) My analysis of data on the Don’t Move Firewood website determined that few of these states regulate firewood. Seven states require treatment of firewood originating out-of-state. New York also prohibits movement of firewood within the state over distances exceeding 50 miles. Two states regulate firewood originating in location quarantined for a specific pest, e.g., EAB. Three states restrict movement of outside firewood onto state properties. The rest of the states urge people to “burn it where they buy it” but impose no requirements. In some cases, National parks for forests have more stringent regulations. I am quite disappointed how few states have taken protective actions. Drake et al. (2026) explained the absence of regulations in the other 11 states as possibly due to the slow pace of legislative action compared to the speed of spread. I think this factor deserves greater attention.

Drake et al. (2026) noted that there are cooperative programs that cross jurisdictional boundaries; these increase programs’ effectiveness. The example they cite is the Ash Protection Collaboration Across Wabanakik — a cooperative effort among federal, state, and tribal governments and non-governmental organizations in northern New England and bordering Canadian and tribal lands.

The discussion of feral pigs reported that these animals are becoming increasingly troublesome. The highest density of pig populations is in southern states but suitable habitat is found across North America. Twelve states have adopted relevant policies; five were proactive in doing so. Feral hogs are present in at least three of the nine states that lack any policy; they are also present in neighboring states of most. Drake et al. (2026) say that the patchwork of policies and regulatory agencies across (and even within states) has hindered management. One of the issues with feral hog management is the presence of conflicting views and stakeholders. Some states encourage hunting, others outlaw it in hopes of reducing any motivation to transport hogs to new areas to initiate sport hunting. They conclude that prohibiting private landowners from profiting from feral pig hunting opportunities, while apparently useful for control, might not be reasonable.

Drake et al. (2026) notes that there is no national policy but the federal government does provide financial assistance. Congressional legislation created the Feral Swine Eradication and Control Pilot Program (FSCP), co-managed by USDA Natural Resources Conservation Service and APHIS. They say that while federal and state investment is likely necessary to conduct the large-scale control needed, the public wants the opposite: they say those responsible for pig releases and individual landowners should pay for control efforts. Drake et al. (2026) discuss the situation in North Carolina to illustrate the conflicting approaches within one state.

Drake et al. (2026) find the greatest consistency across states in the regulation of invasive plants. This might reflect the historical attention to agricultural weeds. However, there are still inconsistencies that might cause confusion and facilitate unintended spread of invasive plants by the horticultural trade. (See my earlier blog here.) They point out that the lack of attention to invertebrates and vertebrates falls short considering the risks and costs these invaders impose at the national and global levels. In the eastern United State, five of the six costliest invasive species are invertebrates; the sixth is feral hogs.

Drake et al. (2026) worry that the widespread differences in approach leads to inaccurate estimates of invasive species’ economic cost as well as reduces states’ ability to effectively plan and coordinate efforts. They concede that given the range of agencies and industries that contribute to invasive species management, their review of state policies might not accurately reflect the full effort. Also the engagement of multiple players enhances flexibility. However, the disconnect between policy and on-the-ground actions can be a barrier to effective communication and compliance. It might also result in duplication and missed opportunities for collaborative management on common goals in neighboring states.

Drake et al. (2026) concede that social acceptance affects implementation. The most cost-effective, efficient, and impactful control methods might be socially unacceptable. Often social acceptance comes after an invasive species has spread and established – so after counter action is most successful and cost-effective.

Drake et al. (2026) note that climate change is likely to reduce barriers to invasive species’ spread and establishment and facilitate transition of benign non-indigenous species into damaging invaders. They say there is an urgent need for more attention from policymakers to the threat posed to both the economy and ecological systems. Their example is the contrast between the concentration of forest insect pests in the northeast while Florida and Mississippi list the highest number of species. Drake et al. (2026) suggest these listings reflect the region’s forestry sector’s concern about non-native pests – but I have not seen such interest (See profile of Sirex woodwasp here.)

To reduce vacillations in federal policy when administrations change, Drake et al. (2026) urge Congress to adopt strong, overarching legislation. If that isn’t possible, they say the second best option is to strengthen incentives and procedures for interstate cooperation. Such an approach could be extended to Canadian provinces

Drake et al. (2026) say it is clear from their own and others’ work that current policy tools fall short and leave proactive states at risk of threats from their neighbors. A possible model is competitive and non-competitive State Wildlife Grants program managed by the U.S. Fish and Wildlife Service. These funds should complement, not be reallocated from, current conservation efforts.

They praise some efforts by NISC, specifically the Early Detection Rapid Response framework, as a way to spur improved communication among policymakers, practitioners, and researchers. However, given the many remaining legislative and regulatory gaps, and differing interpretations, they suggest increasing opportunities of practitioners to use existing research and outreach structures e.g., Land Grant institution extension model. New frameworks such as translational invasion ecology can improve identification of research priorities and transfer of generated knowledge. These frameworks explicitly take into account the ecological, sociological, economic, and political contexts. Incorporating diverse stakeholders and quantitative tools e.g., through simulations, climate change projections, connectivity assessments, and species distribution maps that take into account the socio-economic components might be able to more holistically evaluate and act upon the potential threats.

Drake et al. (2026) call for increased attention to researching species likely to become problematic in the future. They note that only four of 18 NIS species in New England identified by another’s study as likely to benefit from climate change are included under policies of at least one state in the region.

SOURCE

Drake, J., E.M.X. Reed, D. Haak, B. Brown, M.C. Mims, M.G. Sorice, H. Rogers, S. Salom, T. Schenk, and J.N. Barney. 2026. State Lines and Species Divides: Inconsistencies and Opportunities in Invasive Species Policies across the eastern United States. Ecological Applications 36(5): e70287. https://doi.org/10.1002/eap.70287

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Scientific consensus building: international phytosanitary system is failing, needs to be overhauled

The international movement of plant material, particularly plants for planting, is widely acknowledged as a principal driver of the global eruption of forest health epidemics (Brasier, 2008; Turbelin et al., 2017; Tanney et al. 2025; Burgess and Wingfield 2026). The international plant health (or phytosanitary) community in 2012 adopted ISPM#36, with the goal of reducing pest and pathogen introductions on nursery stock. (“Plants for planting” is the regulatory term for this stock.)  However, the top pages of the International Plant Protection Convention’s (IPPC) website do not mention either this issue or the IPPC’s response – this international standard!

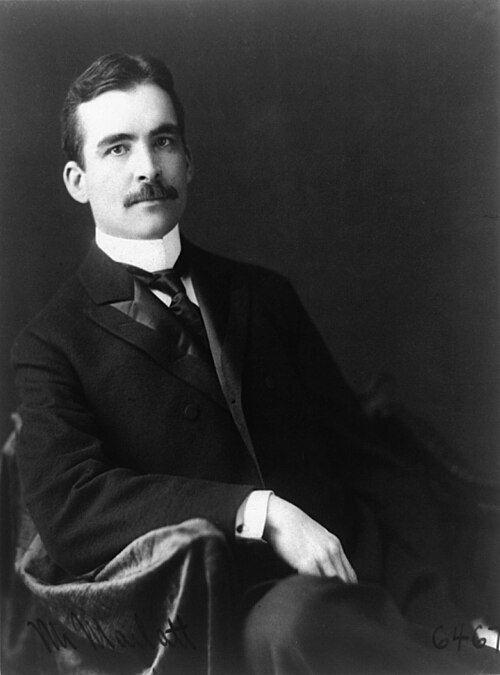
Charles L. Marlatt

Actually, awareness of this risk dates to the 19th Century, at least in Europe. USDA entomologist Charles Marlatt campaigned for the United States to impose phytosanitary rules beginning in 1911. He published a bulletin warning that the U.S. had become a “dumping ground” for contaminated nursery stock from Europe and urged the Congress to act. Marlatt is most famous for requiring destruction of diseased cherry trees sent as a gift by Japan.  Liebhold and Griffin, in their summary of these events,  do not comment on the fact that Marlatt acted without Congressional authority, although destruction of the cherry trees received permission from President Taft. Diplomatic exchanges resulted in Tokyo sending a new batch of pest-free cherries – their descendants grace the Tidal Basin and other parts of Washington, D.C. to this day. At Marlatt’s urging, and following realization of the damage caused by white pine blister rust, Congress adopted the Plant Protection Act in 1912.

This shows that it is possible to protect America’s flora while still enjoying imported plants. But this requires prompt and decisive action, well-prepared in advance, without the likelihood of legal challenges.

Pathogen and Pest Invasions Are Predictable Outcomes

Tanney et al. (2025) say it this way: “We trade not just in plants but also in phytobiomes.” [The phytobiome is the community of microorganisms living on and within a plant.] Burgess and Wingfield (2026) pronounce that invasions are not anomalies but rather predictable outcomes of global commerce interacting with ecological susceptibility. The global nursery trade creates extensive networks that enable the continuous exchange of live plant material across continents. Unlike many others, Burgess and Wingfield (2026) focus not on ornamental horticulture but the repeated occurrence of devastating outbreaks in Eucalyptus and Pinus plantations across the Southern Hemisphere.

Despite a century of efforts to curtail harmful introductions and 70 years after formation of the IPPC, devastating arthropods and disease pathogens continue to be introduced.

Burgess and Wingfield (2026) list the following 11 pathogens introduced since the turn of the 20th Century: Cryphonectria parasitica, Cronartium ribicola, Ophiostoma ulmi/Ophiostoma novo-ulmi and the nematode Bursaphelenchus xylophilus (pine wilt), Phytophthora ramorum, Hymenoscyphus fraxineus, Harringtonia lauricolia, ōhiʻa or myrtle rust (Austropuccinia psidii), and rapid ʻōhiʻa death (Ceratocycstis lukobia and huliohula).

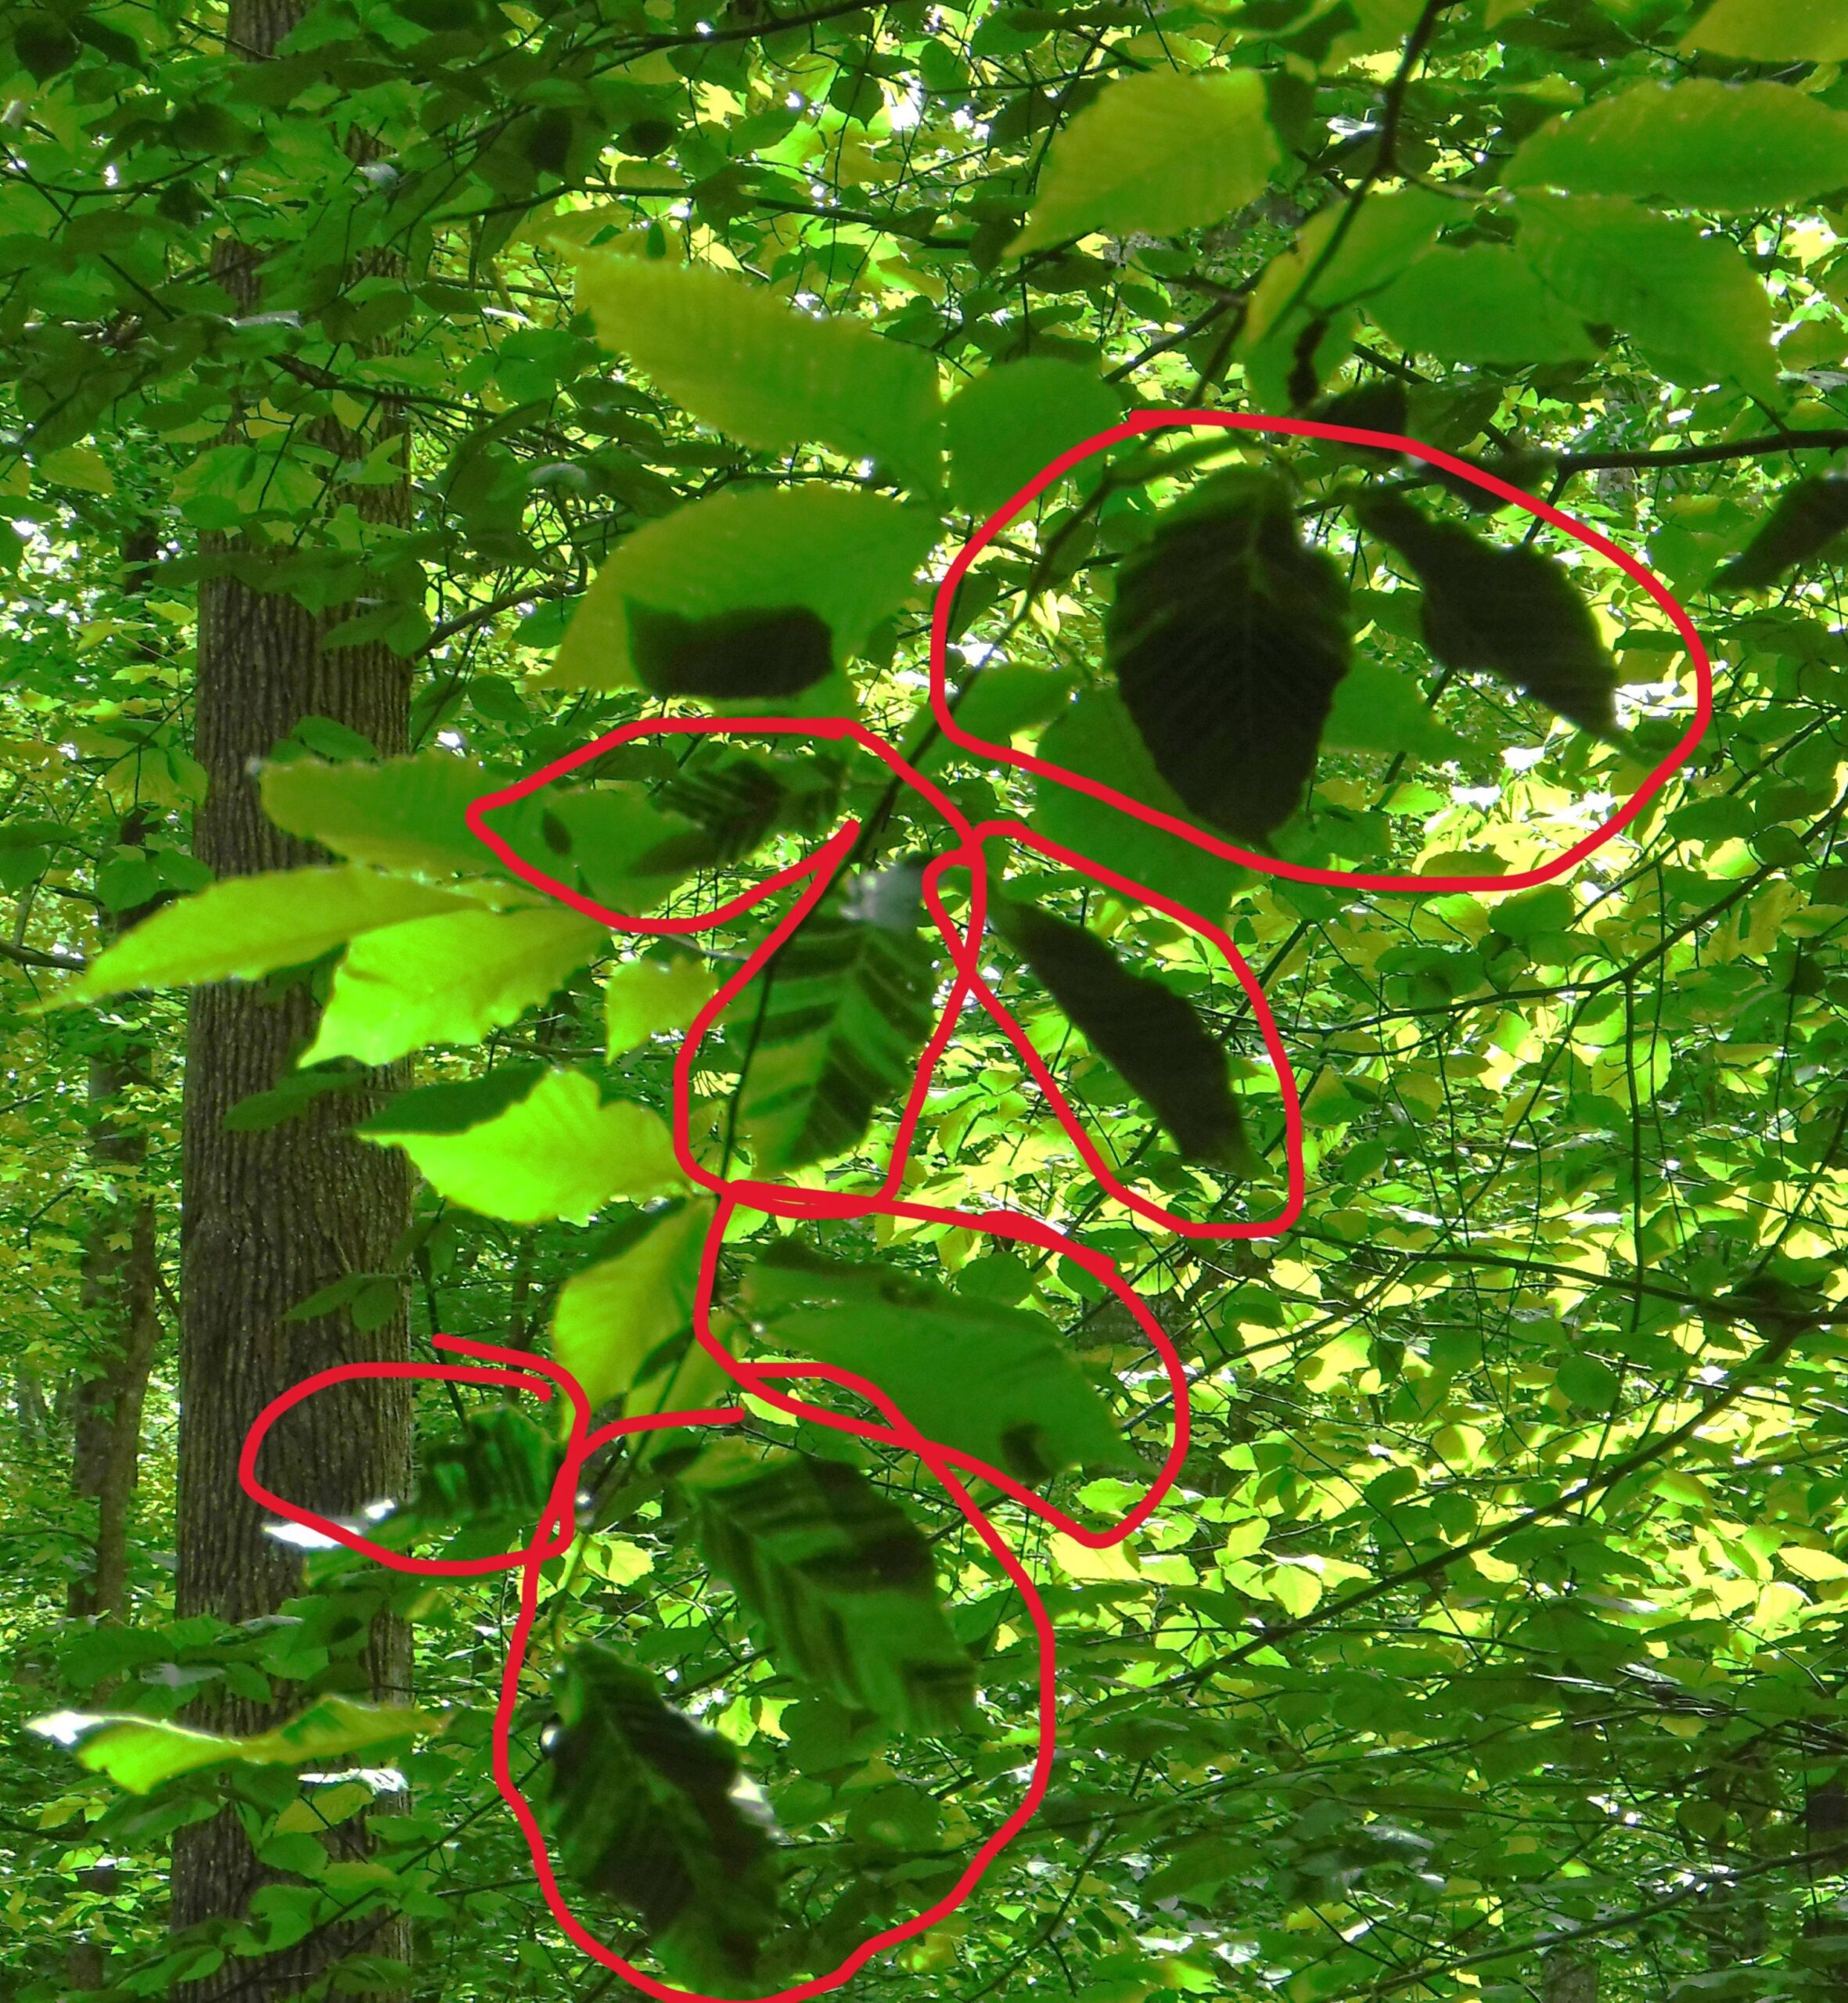
beech leaf disease symptoms, Fairfax County Virginia; photo by F.T.

To this list, I add beech leaf disease nematode (Litylenchus crenatae mccannii), the Euwallaceae/Fusarium complex, and, in Europe, lawson cypress root disease, along with numerous arthropods. These include emerald ash borer (Agrilus plannipennis), goldspotted oak borer (Agrilus auroguttatus), Erythrina gall wasp (Quadrastichus erythrinae). All have irreversibly shaped forest ecosystems in their introduced ranges. The forest losses have had numerous repercussions to human societies in the receiving regions.

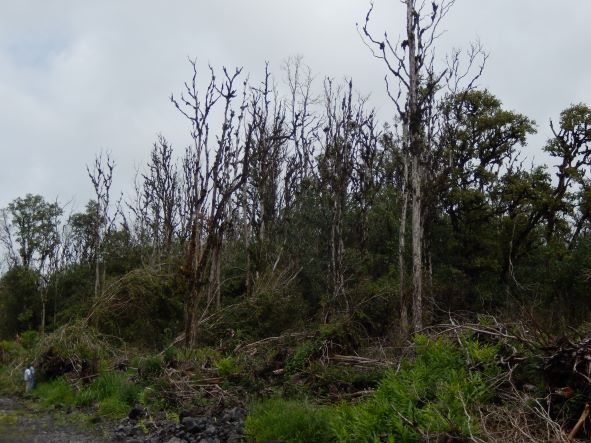
ohia trees killed by rapid ohia death; photo by Richard Sniezko, USFS

Mitigation Can’t Keep Up Due to System Failures

Tanney et al. 2025 opine that the inevitable conclusion is that past and current mitigation efforts have been insufficient to keep pace. Nor do the failures result only from growing volumes of imports that overwhelm inspection services.

They point to another reason: limited acknowledgment and integration of phytobiome-associated risks into regulatory frameworks. The system ignores particularly fungal endophytes and latent pathogens with extended asymptomatic or presymptomatic phases.

Their telling illustration is the ash decline epidemic in Europe. Hymenoscyphus fraxineus is a harmless endophyte–saprotroph on its native Asian host (Fraxinus mandshurica). However, it was introduced to the naïve host European ash (Fraxinus excelsior), on which it became an aggressive necrotrophic pathogen that has killed millions of trees. Even if the organism had been detected (the authors thought this unlikely) before the outbreak was recognized, the detection would not have triggered a risk assessment or any phytosanitary measures. None of the approximately 200 species in the genus had been reported as a pathogen. In fact, a congener, H. albidus, has a similar endophyte– saprotroph life cycle on European ash without causing harm.

McTaggart et al. (2016) flagged these issues a decade ago. They said that recent advances in gene sequencing technologies reveal a vast diversity of fungi causing asymptomatic infections. Some are endophytes, defined as fungi that, for all or part of their life history, asymptomatically colonize plant tissue. Some are pathogens with extended asymptomatic stages. When introduced to naïve hosts, some of either can erupt. Therefore, international phytosanitary measures, including the one significant effort to address the plants for planting pathway, ISPM#36, should focus more on phytobiomes as a biosecurity concern. (See my blog reporting Dr. Eliana Torres Bedoya on this topic.)

Tanney et al. (2025) are not alone in calling out the system’s failure. See Weed, Ayres, and Hicke (2013), Fei et al. (2019), Quirion et al. (2021) for North America; and Gougherty, Sitzia et al. (2021) and Martinac et al. (2025) for a global perspective. Raffa et al. (2023) say national and international phytosanitary policies and programs must reflect the true level of threat from introduced plant pathogens (of all Phyla and Kingdoms) and scientific limits.

Experts on ambrosia beetles – insects that have symbiotic relationships with fungi – say the same. Dell, Xu and Chi 2026 call for studies of Euwallaceae fornicatus’s broader phytobiome, especially bacterial communities, which are increasingly recognized as important components of the ambrosia beetle system.

Nor are Tanney et al. (2025) alone in calling on phytosanitary officials to stop using methods known to fail. That is, relying on visual inspections of plants and basing decisions on whether a pest has previously been designated.

A decade ago McTaggart et al. (2016) called for shifting from a name-based to a gene-based biosecurity risk mitigation approach. Burgess and Wingfield (2026) say officials must move beyond case-by-case responses to embrace broader preventative approaches that address the underlying mechanisms of pathogen emergence and spread.

As Tanney et al. (2025) and Bonello describe, the current international phytosanitary framework relies on symptomatic hosts carrying named pathogens. This approach ignores the facts:

  1. endophytes and latent pathogens with prolonged asymptomatic phases are
    1. ubiquitous – on and in leaves, buds, inflorescences, fruit, seeds, xylem, phloem, cambium, and bark. Phytobiomes are more species-rich on plants lacking disease symptoms.
    1. diverse – fungi, bacteria, viruses, nematodes. Some are known pathogens.
    1. challenging to identify. They often can’t be isolated using standard lab processes. If the genome has not already been sequenced and recorded in databases even sequencing-informative loci or barcodes might fail to identify the taxa. (Only ~150,000 species of an estimated 2.5 million fungi are so compiled.)
    1. in some cases, a significant threat to forest health when introduced to naïve realms.
  2. Scientists cannot predict impacts that might accompany introduction of nearly any of these organisms to a naïve host. Missing information pertains, inter alia, to endophyte identities and life histories, trees’ defenses, and the effects of the current and changing climate.
  3. Host ranges might shift during an organism’s life cycle, e.g., juvenile vs. mature/reproducing.
  4. Host jumps within the same host genus are likely (Tanney et al. 2025). They say that importing living plant into areas with congeneric endemic plants is highly risky.
  5. Most endophytes in woody plants can be horizontally transmitted by abiotic (e.g., wind, rain, and surface water movement) transmission and biotic (e.g., insect) vectors. Every colonized leaf might be a propagule! (Tanney et al. 2025)
  6. Microbes might reproduce both asexually and sexually. Sometimes dispersal of these propagule uses different modes, e.g., insect- and water-dispersed asexual spores combined vs. air-dispersed sexual spores.
  7. Endophytes can switch from being asymptomatic to pathogenic when hosts are stressed. Tanney et al. (2025) name several examples, including Fusarium circinatum – causal agent of pine pitch canker.

To protect our plant resources – in forests, in agricultural fields, in our gardens – scientists must be empowered to develop methods and policies that better account for unnamed and unknown organisms.

Tanney et al. (2025) note that there is some flexibility in the face of unknown threats. The World Trade Organization’s Agreement on the Application of Sanitary and Phytosanitary Standards (SPS Agreement) and ISPM#2 allow adoption of a temporary phytosanitary measure based on the information available, even when it is limited. APHIS’ NAPPRA program link takes this approach. I think countries could use this flexibility more often. (I discuss the SPS and IPPC system in greater detail in my report Fading Forests II. I provide a link at the end of this blog.)

How to Improve Prevention

Some progress has been made in countering introductions of arthropods. Adoption of ISPM#15 regulates an entire pathway (crates, pallets, and other forms of packaging made from wood). CISP applauds the approach but calls for more aggressive enforcement. (On this website, scroll down below “Archives” to “Categories”, click on “wood packaging”). I note that introductions via this pathway nevertheless continue: Lantschner et al. (2026) have identified seven independent introductions of Euwallacea fornicatus. Introductions to San Jose, California; Israel; South Africa; Brazil; Spain; and Türkiye occurred after most countries had begun implementing ISPM#15. The same is true of the introduction of the congener E. kuroshio to southern California. Nardi et al. (2026) demonstrate continuing introductions of woodwasps in wood packaging.

Unlike wood products, imported plants, especially those intended to be planted in the new location, must remain alive and healthy. It is extremely challenging to devise effective treatments to kill the arthropod or pathogen without harming the plant. Tanney et al. (2025) discuss the pros and cons of several options, including ionizing radiation, fungicide treatments, and various heat treatments. They note that more research is needed to assess the feasibility, efficacy, optimal dosage, and potential risks of devitalizing plants in high-throughput treatments.

New Tools for Prevention

So the focus remains on preventing introductions. Fortunately, new tools make possible new approaches.

Detection of Pathogens — Tanney et al. (2025), Carnegie et al. (2026), Burgess and Wingfield 2026, and Bonello (pers. comm.) point to the suite of new molecular, remote sensing, and artificial intelligence tools becoming usable for detecting pathogens. They and Dell, Xu and Chi (2026) stress that citizen science can extend the reach of formal surveillance.

Rapid Responses — Tanney et al. (2025) and Carnegie et al. (2026) concede that more work is needed to address such considerations as detecting DNA from nonviable cells, and to develop international standards. However, they assert that results from these tools are already sufficiently science-based to inform decision-making, specifically to implement rapid responses including precautionary quarantines and other measures along with intensive surveys and conducting triage assessments.

Inspection and Enforcement — Burgess and Wingfield (2026) call more generally for enforcing comprehensive phytosanitary treatments and certifications for the live plant and timber trades, and focusing inspection efforts on high-risk entry points. Port detection can be sped up and improved by applying rapid molecular diagnostic tools.

Risk Assessments — New tools and approaches can also improve risk assessments. I blogged earlier about advances in predicting which trees are likely highly damaged, if certain pest insects are introduced. See Mech et al. 2019; Raffa et al. 2023; Schulz et al. 2025; Uden et al. 2022. This is encouraging, although additional work on arthropods is still needed. Carnegie et al. (2026) and Hulcr (2026, USDA Interagency Symposium on Invasive Species, Annapolis Maryland) both note the need for continued investment in taxonomic surveys to generate baseline data.

Predicting the probable impacts of introduced pathogens is inherently more difficult.

  • After introduction to novel systems pathogens sometimes evolve rapidly and becoming more aggressive and difficult to manage (Burgess and Wingfield 2026).
  • Host jumps within the host genus are likely. This exacerbates the risk arising from importing living plants into areas with congeneric endemic plants. Under these circumstances the risk assessment must be especially careful in balancing economic and social benefits of trade w/ potential ecological, economic, and social consequences of invasion (Tanney et al. 2025; Burgess and Wingfield 2026). Tanney et al. (2025) recommend systematic studies of regularly traded species from areas of origin (or sites of production) to eventual destinations to provide a foundation for assessing the risk of phytobiomes arriving on imported plants. These studies would also help to determine effectiveness of management approaches.

A number of authors are exploring how to address these difficulties. For example, Tanney et al. (2025) advise using “omics”-based approaches to predict invasiveness, virulence, and host interactions. Caveat: same genes are present regardless of whether the organism is an endophyte on its native host or a pathogen on a naïve host. At the same time, host response must be assessed by combining omics-based approaches, sentinel plantings, and modeling.

Tanney et al. (2025) also recommend greatly expanding sentinel planting-based surveillance.  Sentinel plant systems must be carefully managed to provide the necessary levels of information. Raffa et al. (2023) nivemdiscuss strengths and weaknesses of this approach. Eliana Torres Bedoya and Enrico Bonello blog warn that sentinel plantings must support screening all plant parts, above and below-ground, for all potentially pathogenic taxa, including nematodes, phytoplasmas, and viruses. Furthermore, samples must be analyzed from asymptomatic plants, not just those showing signs of disease. Finally, samples must be collected throughout the year. Carnegie et al. (2026) call for greater coordination within the country and with international colleagues (e.g., through the International Plant Sentinel Network (IPSN).

Tanney et al. (2025) provide a convenient list of approaches they think will help close the knowledge gaps that challenge integrating attention to phytobiomes into phytosanitary decision-making.  

Tanney et al. (2025) and Burgess and Wingfield (2026) advocate shifting the focus of risk assessments from specific pests to commodity-based or pathway risk assessments that consider unknown but plausible threats.

Horizon scanning is often described as helpful in predicting the next invasion. However, I have been disappointed by the usefulness demonstrated by some applications of the approach – at least in the absence of policies and resources to support a robust “rapid response”. At least in Cyprus blog and the United Kingdom, the main response to detection of one of the predicted species is only heightened monitoring — not attempted management!! According to Peyton et al. (2026), the British exercise failed to evaluate 78% of the 112 species that were introduced over the following decade. The vast majority were not evaluated because they were expected to have negligible impacts on biodiversity in Britain — but some turned out to be damaging.

Countries also need current data on which to base analyses and determine efficacy of programs. I regret that all American analyses of the risk associated with imported “plants for planting” rely on data collected by Liebhold et al. (2012) — which is from 2009!! Not only are these data 17 years old; APHIS has made major changes to its regulations in the interval — including implementation of the NAPPRA program.

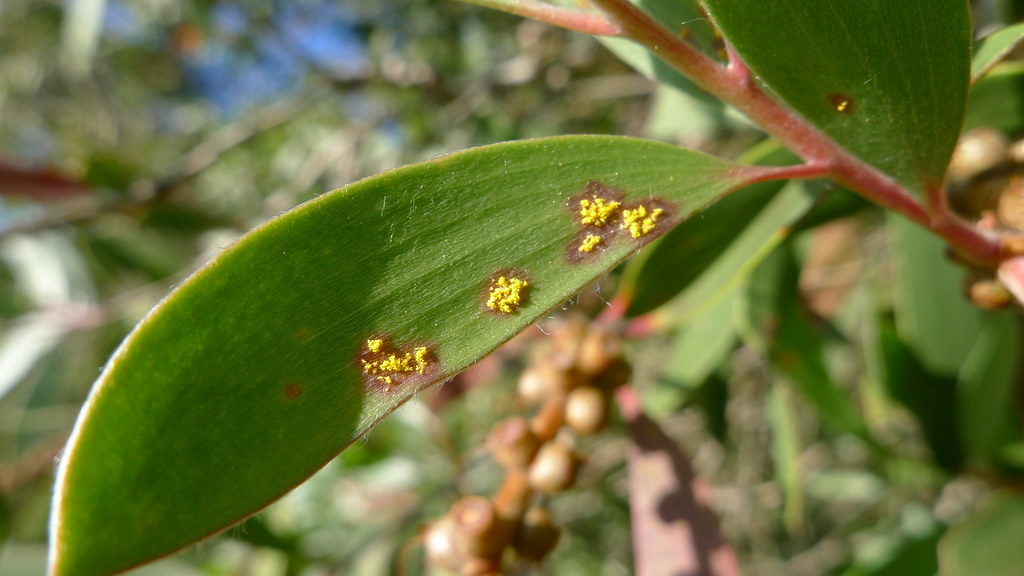
The missing component often is rapid response – often justified by uncertainty regarding the introduced organism’s possible impacts.Wingfield and Burgess (2026) cite the example of Australia’s weak response to detection of myrtle rust, Austropuccinia psidii. Now established in the rainforests of eastern Australia (states of New South Wales, Queensland, and Victoria) and an outbreak in Western Australia, myrtle rust threatens at least 76 species. Australia is home to 38% of all species in the vulnerable Myrtaceae family (Carnegie et al. 2026).

myrtle rust on Melaleuca tree in Australia; photo by John Tann via Flickr

Burgess and Wingfield (2026) cite several lessons based on the Northern Hemisphere’s experience with pathogen introductions. They call specifically for more stringent phytosanitary standards, advanced diagnostic techniques, and risk-optimized surveillance. These should be backed up by collaborative resistance breeding programs for high-risk hosts. They note the need for international cooperation across science, policy, industry, and communities.

Proposed Amendments to Trade Regulations

Tanney et al. (2025) point to the value of shifting to a system that favors trading in propagative material with subsequent bulking up in the importing countries for domestic consumption. (See also my advocacy in Fading Forests II.) They concede that this approach is unlikely to be implemented. As a fallback, they suggest applying this approach to the highest-risk commodities, e.g., rhododendron plants. They note that these plants have transported Phytophthora ramorum.

Scientific Fields

Burgess and Wingfield (2026) point to the need for multidisciplinary research to integrate forest pathology with chemical, ecological and social sciences to anticipate pest emergence. I add: integrating plant pathology with invasion science. The two disciplines rarely interact. Paap et al. (2020) suggest a framework to bridge this gap. I noted that the recent IUCN survey regarding the need for an updated species conservation strategy, while it incorporates invasive species issues, did not mention regional phytosanitary organizations, such as EPPO or NAPPO, among the bodies with whom invasions scientists should build relationships.

Interestingly, a group of experts on invasive plants (Hulme et al. 2026) are trying to expand relationships among researchers even more broadly. They seek to integrate invasion science into on-going discussion of global megatrends. Megatrends are clusters of interdependent global trends observed today that together have the potential to cause significant shifts in environmental, economic, and social conditions. At present, government, industrial, and other leaders evaluating how societies might adapt to these changes are not even considering their probable effect on bioinvasions. At least bioinvasion scientists are starting to evaluate the effects of the megatrends.

The invasion scientists explored how 15 megatrends might affect arrival, establishment, spread, and impacts (environmental and economic) of invading non-native plants over the next 25 years. They grouped the trends into four larger gigatrends: “Anthropocene”, “Digital”, “Societal”, and “Technology”.

They expect most of the megatrends to increase invasion risks, especially by accelerating species arrival and spread. While trends grouped under “Technology” promise some improvements in detection and control tools, there are significant barriers to their adoption. This worrying statement should be addressed by the proponents of applying these measures I cited earlier.

Hulme et al. (2026) urge invasion scientists to persuade policymakers that by taking decisive action to steer these trajectories toward mitigating the growing global threat of bioinvasion.

The Need for Adequate Funding and Political Support

Burgess and Wingfield (2026) note that risk assessment, inspection, detection, and response programs need to be supported by investment in quarantine infrastructure, diagnostic laboratories, and emergency response funds to enhance readiness for new incursions.

As they stress, prevention and preparedness cannot rest solely with scientists. Political commitment, regulatory authority, and industry engagement are indispensable. The efforts need the active participation of affected economic sectors, and sustained investment by governments, scientific institutions,  industry, and society. The need for reliable, long-term funding and societal support is shared with all invasive species programs. Nearly all participants in the IUCN survey ranked this need at the top.

Property owners, the wood products and nursery industries, and governments from municipal to national have incurred substantial economic costs. Entire wooded ecosystems have been destroyed. Affected stakeholders, however, have not demanded that officials adopt more effective plant health  strategies to reduce this risk. Scott Schlarbaum and I have released three “Fading Forest” reports trying to make this happen (links provided below). As shown here, many scientists are calling for action. To quote the late Congressman John Lewis in the context of civil rights, “If not now, when? If not you, who?”

SOURCES

Burgess, T.I. and M.J. Wingfield. 2026. Unveiling a Hidden Menace: Invasive Tree Pathogens, Less Known but Increasingly Threatening Southern Hemisphere Forests Annual Review of Phytopathology 64:18.1–18.2664:18.1–18.26

Carnegie, A.J., B.A. Summerell, C. Trollip F. Tovar, D.I. Smith, and J. McDonald.  2026. Sentinel trees for early detection of non-native forest pests and pathogens in Australia. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Dell, B., W. Xu, and N.M. Chi. 2026. Polyphagous Shot Hole Borer, a Global Threat to Forest Plantations, Green Infrastructure, and Biodiversity: Status, Challenges, and Solutions. Forests, 17, 832

Fei, S., R.S. Morin, C.M. Oswalt, & A.M. 2019. Biomass losses resulting from insect & disease invasions in United States forests

Gougherty, A.V. & Davis,T.J. (2024) Evolutionary history of host trees amplifies the dilution effect of biodiversity on forest pests.  PLoSBio. 22(2):e30024730 https://doi.org/10.1371/journal.pbio.3002475 PLOSBiology |https://doi.org/10.1371/journal.pbio.3002473 February 27, 2024 1 / 1

Hulme, P.E., J.N. Barney, J.L. Bufford, J.A. Catford, J.A. Coetzee, C.C. Daehler, M.S. Dechoum, H. Jäger, A.  Pauchard, P. Pyšek, D.M. Richardson, M. Vilà, E. Wandrag, J.R.U. Wilson. 2026. Seeds of change: Global megatrends will shape the future trajectory of plant invasions. BioScience , 2026, https://doi.org/10.1093/biosci/biag096

Lantschner, M.V., E. Ceriani-Nakamurakare, A.J. Johnson, A.I. Cognato, S.M. Smith, D.F. Gomez. 2026. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis (Coleoptera: Scolytinae), two global emerging pests. J Pest Sci 99, 100 2026. https://doi.org/10.1007/s10340-026-02070-w

Liebhold, A.M., E.G. Brockerhoff, L.J. Garrett, J.L. Parke, and K.O. Britton. 2012. Live Plant Imports: the Major Pathway for Forest Insect and Pathogen Invasions of the US. www.frontiersinecology.org

Martinac, M-L., F. Ningre, A. Dowkiw, N.Le Goff, B. Marcais. 2025.  High host density favour ash dieback. Plant Pathology 2025, 74 (5)  10.1111/ppa.14099

Martinou, A.F., J. Demetirou, I. Angelidou, N. Kassinis, A. Melifronidou, J.M. Peyton, H.E. Roy, A.N.G. Kirschel. 2026. Multiple introductions of invasive alien species on a Mediterranean island predicted by horizon scanning. Biological Invasions 2026 28:41 https://doi.org/10.1007/s10530-025-03729-8

McTaggart, A.R., M.A. van der Nest, E.T. Steenkamp, J. Roux, B. Slippers, L.S. Shuey, et al. (2016) Fungal Genomics Challenges the Dogma of Name-Based Biosecurity. PLoS Pathog 12(5): e1005475. doi:10.1371/journal.ppat.1005475

Mech,  A.M., K.A. Thomas, T.D. Marsico, D.A. Herms, C.R. Allen, M.P. Ayres, K.J. K. Gandhi, J. Gurevitch, N.P. Havill, R.A. Hufbauer, A.M. Liebhold, K.F. Raffa, A.N. Schulz, D.R. Uden, & P.C. Tobin. 2019. Evolutionary history predicts high-impact invasions by herbivorous insects. Ecology & Evolution 9(21): 12216–12230. https://doi.org/10.1002/ece3.5709

Nardi, D., K.E. Wagner, S.F. Ward, A.M. Liebhold, E.G. Brockerhoff, R.M. Turner, J.J. Riggins. 2026. Global movement of woodwasps (Hymenoptera: Siricidae) inferred from border interception records Biol Invasions (2026) 28:167 https://doi.org/10.1007/s10530-026-03881-9

Paap, T., M.J. Wingfield, T.I. Burgess, J.R.U. Wilson, D.M. Richardson, and A. Santini. 202 Harmonising the fields of invasion science and forest pathology NeoBiota Vol 62 2020 pages 301-332

Peyton, J.M., S. Rorke, D.C. Aldridge, O.L. Pescott, K. Dehnen- Schmutz, D.G. Noble,  J. Sewell, A.J.A. Stewart,  T. Adriaens,  B.C. Beckmann,  J. R. Britton, J. Brodie1, P.M.J. Brown, I.C.N. Cavadino, P.F. Clark, A.M. Dunn, J.Foster, C. Harrower, M.C. Harvey, M.C. Jackson, T. Jones, C.A. Maggs, G. Martin, F. Mathews, A.C. Mill, D. Murphy,  E. Paganini, R. Payne, W. Rabitsch, T. Renals,    K. Schönrogge, R.H. Shaw, G.C. Smith, P.D. Stebbing, P.A. Stroh, H. Tidbury, E. Tricarico, J. Vallet,   K.J. Walker, L.E. Wood, C.A. Wood, B. Woodcock, H.E. Roy. 2026. Assessing the success of a horizon scanning approach in predicting invasive non-native species arrival. J Appl Ecol. 2026; 63: https://doi.org/10.1111/1365-2664.70217

Quirion BR, Domke GM, Walters BF, Lovett GM, Fargione JE, Greenwood L, Serbesoff-King K, Randall JM & Fei S (2021) P&P Disturbances Correlate With Reduced Carbon Sequestration in Forests of the Contiguous US. Front. For. Glob. Change 4:716582.  [Volume 4 | Article 716582] doi: 10.3389/ffgc.2021.716582

Rabaglia, R.J., S.A. Dole, and A.I. Cognato. 2006. Review of American Xyleborina (Coleoptera: Curculionidae: Scolytinae) Occurring North of Mexico, with an Illustrated Key. Ann. Entomol. Soc. Am. 99: 1034–1056.

Raffa, K.F., E.G. Brockerhoff, J-C. Gregoirem, R.C. Hamelin, A.M. Liebhold, A. Santini, R.C. Venette, and M.J. Wingfield. 2023. Approaches to Forecasting Damage by Invasive Forest Insects and Pathogens: A Cross-Assessment. Bioscience Vol. 73, No. 2. February 2023.

Schulz, A.N., N.P. Havill, T.D. Marsico, M.P. Ayres, K.J.K. Gandhi, D.A. Herms, A.M. Hoover, R.A. Hufbauer, A.M. Liebhold, K.F. Raffa, K.A. Thomas, P.C. Tobin, D.R. Uden, A.M. Mech. 2025. What Is a Specialist? Quantifying Host Breadth Enables Impact Prediction for Invasive Herbivores Ecology Letters 28: e70083. https://doi.org/10.1111/ele.70083

Tanney, J.B., M. Kemler, M. Vivas, M.J. Wingfield, and B. Slippers. 2025. Silent invaders: the hidden threat of asymptomatic phytobiomes to forest security. New Phytologist 2025 247: 533–545 doi: 10.1111/nph.70209

Uden, D.R., A.M. Mech, N.P. Havill, A.N. Schulz, M.P. Ayres, D.A. Herms, A.M. Hoover, K.J.K. Gandhi, R.A. Hufbauer, A.M. Liebhold, T.D. Marsico, K.F. Raffa, K.A. Thomas, P.C. Tobin, C.R. Allen. 2022. Phylogenetic risk assessment is robust for forecasting the impact of European insects on No Am conifers. Ecological Applications 33(2): e2761. https://doi.org/10.1002/eap.2761

Weed, A.S., M.P. Ayers, J.A. Hicke. 2013. Consequences of climate change for biotic disturbances in North American forests. Ecological Monographs, 83(4), 2013, pp. 441–470

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
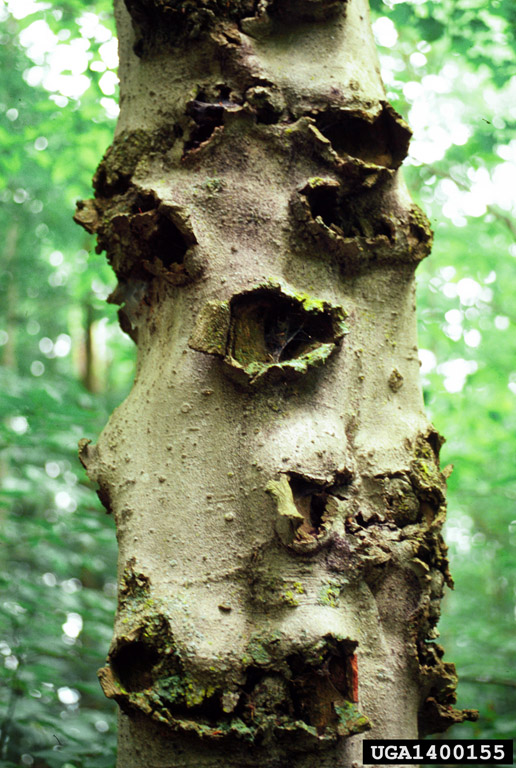
https://fadingforests.org

Southern Hemisphere forests: unique biomes face high invasion risk

native Olia woodiana in forest of Kwa-Zulu-Natal, South Africa. Photo by MJK via Wikimedia

The forests of the Southern Hemisphere faces an elevated risk from introductions of tree-killing arthropods and pathogens. I have already blogged about individual threats to the trees of South Africa, Australia, South America, and Madagascar. This blog will add information about those invasions and provide an overview and call for action.

Burgess and Winfield (2026) [full citation at the end of this blog] – eminent pathologists from South Africa – warn their colleagues that the economic and biological barriers that have long protected the biomes of the Southern Hemisphere from bioinvasion have now collapsed. While these countries remain geographically distant from each other and the Northern Hemisphere, and their floras are certainly still unique, they are now participating in global trade. In addition, they increasingly rely on industrial plantation forestry dominated by non-native tree species – some of them from the North. Finally, climate change is putting additional stress on all these systems.

Burgess and Winfield (2026) advise their colleagues to learn lessons from the alarming history of bioinvasion in the Northern Hemisphere. Over the past century, these forests have been battered by a series of invasions by tree-killing pathogens. They mention the examples we know too well: chestnut blight (Cryphonectria parasitica), white pine blister rust (Cronartium ribicola), “Dutch” elm disease (Ophiostoma ulmi/Ophiostoma novo-ulmi), pine wilt nematode (Bursaphelenchus xylophilus), sudden oak death (Phytophthora ramorum), ash decline (Hymenoscyphus fraxineus), laurel wilt (Harringtonia lauricolia), ʻōhiʻa or myrtle rust (Austropuccinia psidii), https://www.dontmovefirewood.org/pest_pathogen/ohia-rust-html/ and rapid ʻōhiʻa death (Ceratocycstis lukobia and huliohula). They do not address the similarly depressing history of arthropod interchanges among these realms.

Burgess and Winfield (2026) warn that these invasions are not anomalies but rather predictable outcomes of global commerce – especially in “plants for planting” – interacting with the ecological vulnerability arising from the biogeographic similarity of these temperate and boreal forests. The Northern Hemisphere is dominated by a single flora (the Holarctic).

The Southern Hemisphere has an astounding seven floral kingdoms, distributed as follows: Chile-Patagonian, Neotropical, African, Indo-Malesian, Australian, Novozealandic, and Cape. These regions were formerly part of Gondwanaland. Each has an exceptionally high level of endemism (Burgess and Wingfield 2026), but with phylogenic relationships to the flora of other regions. Changing trade patterns are opening introductory pathways for exchange of tree pests hosted by related but geographically distant species. The regional floras’ uniqueness multiplies the conservation importance of protecting them. I summarize Southern Hemisphere countries’ levels of endemism at the end of this blog.

The lessons Burgess and Wingfield (2026) draw from the bioinvasion history of the Northern Hemsphere include:

1) Trade in living plants – and even seeds – creates a high risk that accompanying microbes will be introduced. As noted by others – e.g., Tanney et al. (2025) – members of each plant species’ “phytobiome” are ubiquitous, diverse, difficult to detect, and sometimes capable of causing serious diseases, especially in naïve hosts.

2) After introduction, these microbes can evolve rapidly to adapt to new environments or hosts. They often become more aggressive and difficult to manage in the process. Plant health officials need to anticipate this evolution.

3) Impacts can be catastrophic when a dominant tree species is killed. When chestnut blight killed the vast majority of chestnut trees in North America it destabilized ecosystems and reshaped successional trajectories.

4) The threat is magnified when the receiving ecosystem is a forestry plantation because of the extensive monocultures.   

Building on Burgess and Wingfield (2026) and other sources (where noted), I provide the following summary of threats to native and planted forests in these regions. Some, e.g., Phytophthora cinnamomi and Sirex noctilio, were introduced many decades ago. But too many are recent arrivals.

I. Threats to tree species native to the region.

1) Australia

trees killed by Phytophthora cinnamomi; photo by Western Australia Parks & Wildlife
  • Carnegie et al. (2026) report that more 300 non-native insect pests, pathogens and nematodes are established on tree or shrub hosts in Australia. Twenty percent have caused moderate to high impacts to commercial plantations, urban forests, or trees in natural ecosystems.
  • Phytophthora cinnamomi: As noted, this pathogen was introduced decades ago. It has devastated jarrah (Eucalyptus marginata) forests and diverse plant communities. It causes severe mortality in Proteaceae, Epacridaceae, and Fabaceae. Of ~5700 described plant species in the state of Western Australia, 40% ( >2,300) can be killed (Carnegie et al. 2026).
  • Austropuccinia psidii (myrtle rust): threatens trees in the Myrtaceae worldwide. The rust has spread widely recently, causing severe ecological impacts in invaded regions. The “epidemic strain” introduced to Australia (and other regions) does not infect the commercially important genus Eucalyptus, which probably explains Australian authorities’ lackluster response. However, other lineages of the pathogen found in South America do infect Eucalyptus; introduction of one of these to Australia could be disastrous. Cautionary example of how rapidly a plant pathogen can conquer new ecosystems (Burgess and Wingfield 2026). Already, plant 76 species have been determined to be at risk to myrtle rust. The early focus has been on understory species in the eastern rainforests. Now that myrtle rust has been detected in Western Australia, a biodiversity hotspot with more than a thousand Myrtaceae taxa, most of which are expected to be susceptible. [Summary of Proceedings: Australian Myrtle Rust Conference Sydney, June 2023]
  • Polyphagous shot hole borer Euwallacea fornicatus s.s. (PSHB) and associated pathogen F. euwallacea were detected in 2021, probably three years after it established in Western Australia. Nearly 9% of hosts are regionally indigenous species, 21.3% native to other parts of the continent. There will probably be a considerable impact on the health of conservation reserves & national parks in the future. After trying for four years to eradicate the population, in November 2025, the National Management Group began a transition to a Management Response Plan. This new approach will impose significant additional expenses on local governments and communities for tree removal and replacement (Dell, Xu, & Chi 2026). Meanwhile, the state of New South Wales (2,000 miles away on the other side of the continent) initiated surveillance for PSHB. An assessment determined that 47% of urban trees in Sydney are susceptible to PSHB (Carnegie et al. 2026).
  • Erythina gall wasp Quadrastichus erythrinae (Carnegie and Nahrung 2019). Although Australia is home to at least one native species in the Erythrina genus, E. vespertilio, this pest has not been included on the environmental pest watch list. 

2) New Zealand

native forest on North Island, New Zealand, with kauri tree; photo by F.T. Campbell
  • Kauri dieback / Phytophthora agathidicida is killing Agathis australis, a keystone species that shapes forest structure and has enormous cultural importance for the Maori.

3) South Africa

  • Phytophthora cinnamomi — in the country since 1931 — threatens ecosystem collapse in Cape Floral Kingdom (Burgess and Wingfield 2026).
  • Polyphagous shot hole borer Euwallacea fornicatus s.s. and associated pathogen F. euwallacea The largest outbreak of Fusasrium disease in the world: it is present in every province except Limpopo. The Disease is recorded on 162 tree species. Seventy-eight of these species are indigenous to the country. Eighty-four are “competent” hosts and 78 are “Fusarium colonised” hosts (Townsend, Hill, Hurley and Roets 2025).
  • Fungus Seiridium neocupressi detected on the native tree, Widdringtonia nodiflora year The two other species in the genus, W. wallichii and W. schwartzii, occur in small endemic and threatened populations (Wingfield et al. 2022).

4) Madagascar

  • Leptographium calophylli killing an endemic tree species in mid-level elevation humid and subhumid forests, Calophyllum paniculatum.  

5) South America

  • Polyphagous shot hole borer Euwallacea fornicatus s.s. and associated pathogen F. euwallacea has been detected in Brazil, Argentina, and Uruguay. Dell, Xu, & Chi (2026) report that in Uruguay a significant number of native species are reproductive hosts for the beetle. Models developed by Coates and Philips (2026) indicate PSHB could thrive in more suitable habitats.
  • One of the continent’s native conifers, Austrocedrus chilensis is under attack by both an introduced aphid, Cinara cupressi and the pathogen Phytophthora austrocedri
Chilean cypress; photo by LBM via Wikipedia

Lantschner et al. (2026) identified seven independent introduction events of E. fornicatus: to the continental U.S., Hawai`i, South America, Central Europe, Spain, Türkiye, & South Africa.

II. Threats to plantations:

1) Co-evolved insects and pathogens have followed their Pinus hosts to plantations in the Southern Hemisphere due to biosecurity failures

  • Insects: Sirex noctilio (decades ago); recently Sirex obesus in Brazil (2023); Orthotomicus erosus and Cyrtogenius luteus (Stazione, Soliani, and Cognato 2026).
  • Pathogens: Fusarium circinatum, Dothistroma septosporum, Diplodia sapinea,  Phytophthora pinifolia, Lecanosticta acicula.

2) Because the Myrtaceae family is distributed around the Southern Hemisphere, plantations of Eucalyptus trees are now being damaged by both pathogens from their native Australian range (Teratosphaeria spp.) and local pathogens that have switched hosts (Chrysoporthe cubensis and Chrysoporthe deuterocubensis).

Burgess and Wingfield (2026) express fear that another set of pathogens, rapid ohia death (Ceratocystis lukuohia and Ceratocystis huliohia) might spread from Hawai`i farther across Oceania to New Zealand and other locations with important species in the Metrosideros genus. I note that the more virulent (on ʻōhiʻa) C. lukuohia belongs to an Asian-Australian clade (Luiz et al. 2023).  

Australia

I blogged in November 2022 about how surprising tardy Australia was in implementing phytosanitary programs to protect the nation’s forests. Scientists had spent 30 years trying to get such a program implemented. Burgess and Wingfield (2026) point out that 16 of 17 pathogens detected in Australia over the period 1996 – 2017 had established; several had had major impacts. None has been eradicated. They also note that the introduction of Austropuccinia psidii exposed significant weaknesses in post-border surveillance and response. 

The Australian federal govt has implemented a detection trapping program targeting the Asian spongy moth (= flighted spongy moth complex) at the 4 major ports (i.e., Melbourne, Hastings, Geelong and Portland) since 1996.

Carnegie et al. (2026) describe some helpful steps. They focus on establishment in 2022 of a National Forest Pest Surveillance Program (now called Forest Watch Australia). The program is funded by a levy on forest plantation growers and State governments, based on the relative risk to each region. Surveillance efforts are concentrated in areas deemed high risk areas for entry and establishment of forest pests. Program is coordinated through the federal agency, Plant Health Australia. It provides professional training for surveillance and diagnostic staff on an annual basis. Staff also conduct risk modelling and analysis to identify high-risk areas for surveillance in all major capital cities — Sydney, Melbourne, Brisbane, Hobart, Adelaide, Perth and Darwin.

The Australian program encounters the universal challenges regarding sustained resources, the diagnostic burden placed on scientists, and ownership of data. Carnegie et al. (2026) and Burgess and Wingfield (2026) discuss the growing availability of new tools for detection, e.g., molecular diagnostic tools.

Response options are guided by the national Emergency Plant Pest Response Deed and PlantPlan,  which outlines agreed government and industry responsibilities and cost-sharing protocols.  

Carnegie et al. (2026) praise especially the sentinel tree component of the surveillance program. Participants include governments at the federal, state, and municipal levels; botanical gardens; and industry. In 2024/25, trained staff inspected 5,136 trees of more than 50 species across 45 genera nationwide. Thanks to this expanded effort, the detection rate of new species has doubled since 2018, from ~ 1.5 to ~ 3 / year. Still, in three of four cases discussed by Carnegie et al. (2026), the introduced organisms were determined to be too widespread for eradication to be successful. They cite the PSHB outbreak in Perth as an example. Carnegie et al. (2026) advocate strengthening sentinel tree surveillance in urban landscapes so detection will occur sufficiently early to allow consideration of initiating an eradication or containment response. One worrisome aspect: there is no requirement to conduct more thorough surveillance or diagnostics on a species detected in the country once it has been ruled not “of concern”.

Burgess and Wingfield (2026) advocate embracing broader preventative approaches that address the underlying mechanisms of pathogen emergence and spread. I forthcoming blog will discuss proposed new approaches.

Background: Southern Hemisphere Flora

South Africa

As I blogged recently, South Africa’s flora is diverse (more than 20,000 indigenous species) and has high levels of endemism. That blog did not discuss the Myrtaceae family – my focus now because of the spread of the pathogen Austropuccinia psidii. According to Braam van Wyk and Hugh Glen (pers. comm.), the country has 24 native Myrtaceous species. These include 14 species in the Eugenia genus, six in the Syzygium genus. The one Metrosideros grows in the Cape Floristic Region. All the others occur in forest or grassland along the Indian Ocean Coastline well into Mozambique and further inland – some into Botswana and Zimbabwe.

Australia                      

Australia ranks second on Earth in the proportion of its flora that is endemic: 88% of plants. Australia comprises the native range of 38% of all Myrtaceae species on Earth, and of 66% of genera in the family (Brett Summerell, 2023 workshop). These 87 or 88 genera contain ~ 2,250 species and subspecies (Makinson 2018). This plant family constitutes ~10% of the continent’s native flora. They occur in 11 of 13 major vegetation formations (Carnegie et al.2026). The southwestern corner of Western Australia alone has ~5700 described plant species (Carnegie et al 2026).

Rhodomyrtus psidioides – one of the Australian Myrtaceae under greatest threat from myrtle rust; photo by Zaadero via Wikimedia

The island of Madagascar is home to 12,000 plant species, of which 83% are endemic.

SOURCES

Burgess T.K., and M.J. Wingfield. 2026. Unveiling a Hidden Menace: Invasive Tree Pathogens, Less Known but Increasingly Threatening Southern Hemisphere Forests Annual Review of Phytopathology #s

Carnegie AJ, Summerell BA, Trollip C, Tovar F, Smith DI and McDonald J (2026) Sentinel trees for early detection of non-native forest pests and pathogens in AU. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Ceriani-Nakamurakare, E., Johnson, A.J. and Gomez, D.F. (2023) Uncharted Territories: First report of Euwallacea fornicatus (Eichhoff) in South America with new reproductive hosts records. Zootaxa, 5325 (2), 289–297. https://doi.org/10.11646/zootaxa.5325.2.10

Lantschner, M.V., Ceriani-Nakamurakare, E., Johnson, A.J. et al. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis, two global emerging pests. J Pest Sci 99, 100 (2026). https://doi.org/10.1007/s10340-026-02070-w

Luiz, B.C., C.P. Giardina, L.M. Keith, D.F. Jacobs, R.A. Sniezko, M.A. Hughes, J.B. Friday, P. Cannon, R. Hauff, K. Francisco, M.M. Chau, N. Dudley, A. Yeh, G. Asner, R.E. Martin, R. Perroy, B.J. Tucker, A. Evangelista, V. Fernandez, C. Martins-Keli’iho.omalu, K. Santos, R. Ohara. 2023. A framework for establishlishing a rapid ‘Ohi‘a death resistance program  New Forests 54, 637–660. https://doi.org/10.1007/s11056-021-09896-5

Stazione, L., Soliani, C., Cognato, A. et al. Reconstructing the invasion history of the bark beetles Orthotomicus erosus and Cyrtogenius luteus (Coleoptera, Curculionidae, Scolytinae) in South America. Biol Invasions 28, 49 (2026). https://doi.org/10.1007/s10530-026-03779-6

Tanney, J.B., M. Kemler, M. Vivas, M.J. Wingfield, and B. Slippers. 2025. Silent invaders: the hidden threat of asymptomatic phytobiomes to forest security. New Phytologist (2025) 247: 533–545 doi: 10.1111/nph.70209

Wingfield, M.J. S. Marincowitz, N.Q. Pham, F. Roets, T. Paap, B.D. Wingfield, J. Aylward. 2022. Cypress canker: An important disease discovered for the first time on a native South African tree. Plant Pathology 2022;71:1735-1742

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
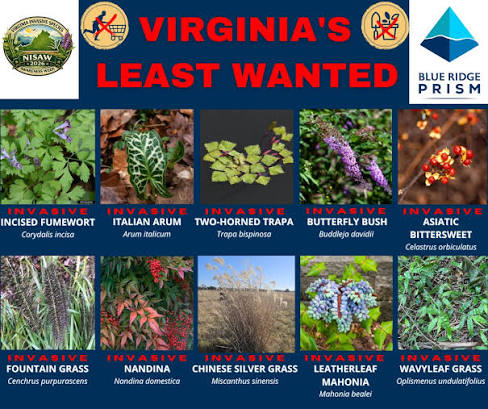
https://fadingforests.org

Tree regeneration update

sycamores overcome by invasive vines, primarily porecelain berry; photo by F.T. Campbell

18 months ago I blogged about the impacts of invasive plant species and deer on regeneration of tree species.  I provide more information on some National Park units’ efforts to counter these threats – contemporaneous with release of the report.

Emma Brentjens has posted a report with pictures. She focuses on National parks in the National Capital Region (NCR). These are the National parks in Maryland, Virginia, and a small part of West Virginia, including Catoctin Mountain Park; Antietam, Manassas, and Monocacy National battlefields; Harpers Ferry and Chesapeake & Ohio National Historical parks; Rock Creek Park; some parkways; and some urban parks, e.g. Anacostia and East Potomac. Forests constitute three-quarters of the landcover in National parks of this region. Regional NPS staff noted poor regeneration as early as 2006. In the years since, most have ramped up IAS plant management, & begun deer population management. As result, the previously steady regeneration declines have begun to reverse.

They analyze forest vegetation data using the Stocking Index, which calculates seedling density per hectare. “Acceptable” forest regeneration is defined as 67% of plots being adequately stocked. Unfortunately – from my perspective – the program accepts non-native tree species as successful regeneration.

Comparing the parks’ Stocking Index in 2006-2009 to 2020-2024 showed that most of these parks have seen an increase in the Stocking Index, including most sites managing deer populations. Still, no parks have yet achieved adequate stocking for more than 30% of the plot.

Most parks that are managing their deer populations show growth in seedling density, e.g., Catoctin Mountain Park (illustrated in the report); Harpers Ferry National Historical Park; and Monocacy National Battlefield. In Rock Creek Park, which also manages deer, many seedlings have grown into saplings.

deer in Shenandoah National Park; photo by F.T. Campbell

Most of the sites with declines in seedling density have not implemented deer management. These include several segments of Chesapeake & Ohio Canal National Historical Park and the parkways. Unfortunately, it also includes Prince William Forest Park, which at 15,000 acres is the largest protected area near Washington, D.C.

Brentjens notes that while these early results are promising, seedling levels are highly variable and do not guarantee forest regeneration. Continued management is necessary to sustain improvements.

As part of deer management, the NP units are also monitoring spread of chronic wasting disease (CWD) among white-tailed deer. Current CWD rates are very low (< 1%). The disease has been confirmed at four parks in the region: Antietam, Manassas, and Monocacy National battlefields and Harpers Ferry National Historical Park.

(Chronic wasting disease is not an effect too to reduce deer populations. First, is relying on such suffering an ethical approach? Second, significant declines in deer populations are not observed until infection rates reach about 29% of the population. Parks in the National Capital Region are not expected to reach that level for at least 20 years.

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Protecting forests’ ecosystem values: minimize disturbance & curtail nearby planting of non-native species

old-growth forest in Tioresta Research Natural Area, Allegheny National Forest (Pennsylvania); photo by Nicholas T via Flickr

The implied or explicit recommendations are not new. But they are supported by new data!

Several measures of forest health drawn from survey plots of the Forest Inventory and Analysis (FIA) show that federally-owned forested lands – in both National forests and National parks – are healthier than neighboring forests under different ownership. Forest inventory plots in federal forests have significantly greater tree species and structural diversity and evenness; basal area and biomass per hectare; and seedling density. They are also less invaded by non-native plants. These findings hold across the continental United States, four regions (North, South, Rocky Mountains, and Pacific Coast) analyzed separately, and 22 common forest types.

The consistent finding of more “mature forest” features in eastern National parks and National forests – regardless of longer-term land-use histories (Potter et al. 2026b) – seems to me to indicate that recent and current management practices might overcome influences of centuries of pre-protection land use histories of exploitation and degradation.

1. Forest Health Inside vs. Outside Federal Forested Lands

Legally designated USFS National forests comprise ~19% of the Nation’s total forest area (~59 million out of 310 million hectares). Since adoption of the Forest and Rangeland Renewable Resources Act of 1974, the National Forest System (NFS) within USDA has been managed to maintain “appropriate forest cover . . . to secure the maximum benefits of multiple use sustained yield management in accordance with land management plans”. The Department of Interior’s National Park Service units are managed to conserve unimpaired the natural and cultural resources and values in the system for the enjoyment, education, and inspiration of this and future generations (National Park Service “Organic Act” of 1916).

Potter et al. 2026b assessed the ability of National forests to provide ecosystem services and forest products in the face of dramatically increasing threats:  (1) more intense and frequent wildfires; (2) uncharacteristically long and hot drought conditions; (3) mortality and compositional changes caused by invasive forest pests; (4) competition from invasive plant species; and (5) forest fragmentation and conversion to other land uses. To do this, they asked whether National forests (1) have greater biodiversity – as measured by species and structural diversity; (2) are denser and encompass more biomass; (3) experience more regeneration; and (4) are less invaded by non-native plants. The FIA surveys were carried out from ~2010 to ~2022. As noted, they analyzed each comparison across the conterminous states, the four regions, and the 22 forest types. 

Potter et al. (2026b) and an earlier study by Miller et al. (2016) agree that ownership determines forest management, specifically the level of anthropogenic disturbance allowed. Miller et al. demonstrated that, in the eastern United States, forests in National parks have greater live tree basal area, a larger volume of coarse woody debris, and greater proportions of late-successional tree species than nearby forests. They also have lower rates of tree growth and mortality.

Potter et al. (2026b) found that all biodiversity indicators except number of saplings per hectare were higher for plots inside the NFS than neighboring forests under other ownerships. This was true across the continent and in all four regions.

In some of the 22 forest types the indicators were particularly strong. Thus, basal area was notably higher on NFS forests populated by loblolly/shortleaf pine, Western larch, hemlock/Sitka spruce, maple/beech/birch, and oak/hickory forest types. Tree species richness was significantly higher on NFS plots for Western larch, elm/ash/cottonwood, longleaf/slash pine, pinyon/juniper, and loblolly/shortleaf pine. Differences in regeneration were seen most prominently in loblolly/shortleaf pine, oak/hickory, oak/pine, and white/red/jack pine. The authors do not speculate on the reasons.

a large loblolly pine in Congaree National Park; via Picaryl

The FIA data showed that invasive plant richness and cover were both greater on plots outside National forests across the Continent and in all four regions. However, invasive plant richness did not differ by ownership for some specific forest types: elm/ash/cottonwood, pinyon/juniper, Western larch, and hardwood woodlands. (National parks are even less invaded by non-native plants than National forests; see below.)

2. Regions Differ – Why?

Geographic regions differed noticeably. Tree species richness and evenness; diversity and evenness of tree height classes; biomass/ha; seedlings and saplings per hectare; and invasive plant diversity and cover were higher in the East – in both USFS Northern and Southern regions. Tree species richness was by far highest in the South – especially in the southern Appalachians and on the Cumberland Plateau. Seedling density was highest in the North, moderately high in the South. In the North, tree species and tree height evenness were both higher on non-federal lands.

Invasive plant richness was highest in some parts of the South. [See a more detailed discussion of invasive plants below.] Tree diameter class diversity and evenness were significantly higher in the West. Basal area was by far the highest in the northern part of the Pacific coast region (Washington, Oregon, and California.). Seedling density was moderately high in some National forests in the Rocky Mountains. Tree diameter evenness was higher outside National forests in the Rocky Mountains.

These differences had been expected given the marked regional dissimilarities in floristic, climatic, and edaphic factors, as well as ownership patterns.

Potter et al. (2026b) report that tree recruitment was stronger in the East than the Rocky Mountain and Pacific coast regions. I wish they had discussed how this finding relates to earlier findings (Potter and Riitters 2022) that numbers of species experiencing poor regeneration were highest in the Southeast, followed by the Northeast and Midwest. Miller et al. (2023) also found that tree regeneration was poor in National parks from Virginia to Maine. The latter study attributed this failure to a combination of browsing by overabundant deer and competition by invasive plants. The latter is presumably even more important in national forests, which are invaded by non-native plants at twice the rate of national parks. Nonfederal forests are invaded at even higher rates – up to 3 times greater. [See here for a study of improve regeneration in National parks which control their deer populations.]

Potter et al. (2026b) note that the higher forest health indicator values for NFS forests prevailed across the Continent despite notable differences in land-use and management histories and landscape contexts. Most NFS land in the West was put under federal management before arrival of European pioneers, so more of their groves are classified as old-growth or mature. In the East, nearly all lands incorporated into the National Forest System were privately owned until they were purchased in the 20th Century. At that time these forests were often highly degraded. Not only did the eastern National forests have to recover from overexploitation; they are still typically embedded in a matrix of other land ownerships, often largely cleared of trees.

In their analysis, Potter et al. (2026b) controlled for differences in site productivity and some environmental conditions e.g., elevation and slope, but not soil or hydrological conditions. So they believe that the suite of environmental factors do not explain the “older” attributes of eastern forests managed by the USDA Forest Service and USDI National Park Service,. These attributes generally include a more complex forest structure; higher tree species richness; and greater basal area and density of live trees (Miller et al. 2016). 

What differs is management. Miller et al. (2016) say explicitly that protection from forest harvesting for many decades probably is an important explanation of why forests in the eastern National parks have greater tree species diversity than forests owned by other parties. Potter et al. (2026b) instead emphasize the impacts of different land-use histories outside of National forest boundaries. Much of this land (especially in the East) has experienced continuous, centuries-long agriculture and residential development and more acute disturbance pressures associated with higher human population density. They also note that managers of non-federal forests goals often call for harvests or other active management – which can reduce forest structure, species richness, size of live trees, presence of downed woody debris, etc.    

I note that the consistent finding of more “mature forest” features in eastern National parks and National forests – regardless of longer-term land-use histories (Potter et al. 2026b) – indicates that recent and current management practices might overcome older influences. Many of these forests have enjoyed protective management for less than a century; the Forest and Rangeland Renewable Resources Act of 1974 was adopted just 50 years ago. I assert that the decisive factor might be the much lower presence – although not absence! – of deliberately planted non-native plant species on federal properties. [Again, see a more detailed discussion of invasive plant issues below.]

Potter et al. (2026b) also comment that regeneration on NFS land is almost exclusively natural. As discussed above, they consider this regeneration to be successful, in that seedlings generally are being produced in greater numbers than on surrounding forests in other ownerships. Again, I would like to learn how this finding relates to the earlier study by Potter and Riitters (2022).

Potter et al. (2026b) state that National forests benefit from their greater size and stability of management goals. These are necessary for large-scale approach to conserve or imitate the processes that create diversity

As Potter et al. (2026b) note, in the East, reserved areas like National forests (or to a greater extent, National parks) represent a small proportion of the landscape. Their distinctness from neighboring forestlands emphasizes their ecological value.  They call for managers to be alert to potential invasions of non-native plants or tree-killing pests from the surrounding agricultural and developed land. In the West, private forests abut federal forested lands less often and thus have less influence on the status of forest health indicators on National forests.

3. Plant Invasions in Forests

Several studies by Kevin Potter, Kurt H. Riitters and colleagues have documented the extent of plant invasions in America’s forests.  Data supporting these studies come from the same forest plot surveys conducted under the Forest Inventory and Analysis (FIA) program.

The region most invaded is Hawai`i: 83% of FIA plots have one or more invasive plant species. The region that ranks second is the East, specifically the 37 states comprising the USDA Forest Service’s former Northern and Southern regions. Nearly 53% of FIA plots in this region have one or more invasive plant species (Potter et al. 2024). FIA plots in the Rocky Mountain West had only 11% (Potter et al. 2026a).

student volunteers in Camp S.E.E.D. (Students Encouraging Environmental Recovery) program pulling invasive plants in Shenandoah National Park; via Picaryl

As noted above, invasive plants are particularly problematic in the South. There, invasive plants have been documented on 55.3 million hectares. In the Northern Region, an incomplete survey found invasive plants on 36.9 million ha. In some counties of the 37 states, 80% of inventoried forest plots contain invasive plants. Spread of these invaders is largely unchecked. The invasions’ extent and intensity are so great that their complete removal – or elimination of their impacts – is “practically impossible” (Potter et al., 2024; Potter et al. 2026a).

Plant invasions in eastern forests are undoubtedly worse than these data indicate because the records include only some of the non-native plant species present — those considered to be the worst invaders at the time regional lists were compiled (Potter et al. 2026a). Not included on the survey list are wavy-leaf basketgrass (Oplismenus undulatifolius), fig buttercup (Ficaria verna), shrub and creeping Euonymus, callery pear (Pyrus calleryana). Only one privet (Ligustrum vulgare) is included.

Furthermore, Bradley, Early and Sorte (2015) report that while non-native plant species are already more widely distributed than native species, the average invasive plant species inhabits only about 50% of its expected range.

Sites Most Heavily Invaded

Analyses of the FIA data reveal several overlapping definitions of which locations and situations have been invaded most severely. These factors are separate from the issue of ownership discussed above. Invasive plants are more numerous, widespread, and diverse in more disturbed or fragmented sites. One study found that 65% of plots that experienced greater fragmentation were invaded compared to 46% of plots that experienced low fragmentation. Invasion rates are highest in the “wildland-urban interface” (WUI). Unfortunately, the WUI is growing faster than any other land use type in the country – especially in the East (Potter et al. 2024). Because the East is so heavily developed, a plot’s distance from a road was nearly irrelevant. Furthermore, development in the WUI also promotes planting of non-native species that might then invade the nearby forest. See my more detailed discussion of these issues here.

Highly productive sites [defined as a site’s ability to grow industrial timber; Potter et al. 2026b] are also prone to invasion: 76% of highly productive plots were invaded compared to 40% of low-productivity plots. It is not known whether highly productive sites are inherently more invasible, or, instead, that such plots were converted to agriculture earlier, so exposed to human disturbance longer (Riitters et al. 2017).

A third analysis found that the best predictor of the odds that a site would be invaded was the site’s ecological province as defined by Robert G. Bailey in 1995 (Riitters et al. 2017)

Propagule Pressure: the Role of Deliberate Planting

Over 25 years (Reichard and White 2001) numerous scientists have documented the role of deliberate planting – especially ornamental horticulture – in facilitating introduction and spread of invasive plants. Kinlock et al. (2025) found that more than 1,600 plant species sold by nursery and seed catalogs over 200 years had “naturalized” somewhere in the continental 48 states. Fertakos and Bradley (2024) found that species were likely to establish if they were introduced to as few as eight locations. Beaury et al. (2023) found that half of 89 plant species recognized as invasive are sold in the same locations where they are invasive. Another 25 species are sold in an area that is currently unsuitable for those species, but that will become more suitable for invasion as temperatures warm.

Japanese barberry – invasive that is widely sold; photo by Matthew Beziat via Flickr

Both Potter et al (2024) and Potter et al. (2026a) note that the flora of suburban and rural residential landscapes is dominated by non-native plant species. I add that the people who live there promote plant invasions in various ways, including planting shrubs or flowers in the woods and dumping yard waste there. The older the human settlement, the more years for these plants to spread – assisted by birds, wind, or water. Go here for a more detailed discussion of these issues.

What Should We Do to Curtail Introduction and Spread of Invasive Plants?

a. Regulations The ornamental plant market – whether brick and mortar stores or internet sales — is interstate in scope. Regulations need to match (Beaury et al. 2023). This requires Congress to adopt a new federal law. Under the Constitution, the appropriate entity for regulating interstate commerce is the federal government. But the current statute (the Federal Noxious Weed Act) does not address long-established, widespread species.

States currently have the lead in regulating sales of horticultural plants. Beaury et al. (2023) and Evans et al. (2024) criticize state restrictions as outdated, limited to a few weeds that plague agriculture, and irregularly enforced. The result is a checkerboard of places where a species is offered for legal sale next to places where that sale is prohibited. Finally, the regulations are reactive; they rarely include plants in anticipation of their spread to new areas. Evans et al. (2024) urge state regulators to prioritize those species in the ornamental trade that are projected to remain or become abundant under evolving climate conditions.

b. Voluntary Actions

Potter et al. (2024) call for efforts to encourage homeowners to plant more native and environmentally friendly private landscapes. They concede the complication that some non-native – even invasive – species provide valued ecosystem and cultural services. They also suggest that local governments adopt land-use planning rules that protect forests of high conservation value. They do not discuss the extreme improbability of the latter action given the magnitude of predicted land-use changes in the country, powerful demographic factors driving them, and lobbying clout of affected economic interests, including the nursery industry.

Many citizen associations – native plant societies, regional or state invasive plant councils, etc. – are pursuing the education approach. (See the websites for state native plant societies, Southeast Exotic Pest Plant Council, Mid-Atlantic Invasive Plant Council, Midwest Invasive Plant Network, and Virginia Invasive Plant Coalition.) These voluntary efforts have yielded some success. But they have not resulted in adequate protection for our ecosystems.

c. Land-Managing Agencies

Many land-managing agencies work with local and regional groups to monitor and remove invasive plants, e.g., Blue Ridge PRISM. Databases that verify and post their findings, e.g., iNaturalist and EDDmapS can provide early warning of new invaders. See here for a discussion of these matters.

Blue Ridge PRISM removing English ivy; photo courtesy of Rowena Zimmerman, Director of Virginia Invasive Plant Coalition & Blue Ridge PRISM

Potter et al. (2026a) also suggest that the USDA Forest Service update the lists of invasive plants to be included in future FIA surveys. I agree. See above for examples of highly invasive species not now included.

Of course, the influence of plants on ecosystems is broader than invasive species. Dr. Douglas Tallamy has demonstrated that even non-invasive, non-native plants can disrupt food webs.

 SOURCES

Beaury, E.M., J.M. Allen, A.E. Evans, M.E. Fertakos, W.G. Pfadenhauer, B.A. Bradley. 2023. Horticulture could facilitate invasive plant range infilling and range expansion with climate change. BioScience 2023 0 1-8 https://doi.org/10.1093/biosci/biad069

Bradley, B.A., R. Early and C. J. B. Sorte. 2015. Space to invade? Comparative range infilling and potential range of invasive and native plants. Global Ecology and Biogeography

Evans, A.E., C.S. Jarnevich, E.M. Beaury, P.S. Engelstad, N.B. Teich, J.M. LaRoe, B.A. Bradley. 2024. Shifting hotspots: Climate change projected to drive contractions and expansions of invasive plant abundance habitats. Diversity and Distributions 2024;30:4154

Fertakos, M.E. and B.A. Bradley. 2024. Propagule pressure from historic U.S. plant sales explains establishment but not invasion. Ecology Letters 2024;27:e14494  doi: 10.1111/ele.14494

Kinlock, N.L., D.W. Adams, W. Dawson, F. Essl, J. Kartesz, H. Kreft, M. Nishino, Jan Pergl, P. Pyšek, P. Weigelt and M. van Kleunen. 2025. Naturalization of ornamental plants in the United States depends on cultivation and historical land cover context. Ecography 2025: e07748 doi:10.1002/ecog.07748

Miller, K. M., F. W. Dieffenbach, J. P. Campbell, W. B. Cass, J. A. Comiskey, E. R. Matthews, B. J. McGill, B. R. Mitchell, S. J. Perles, S. Sanders, J. P. Schmit, S. Smith, and A. S. Weed. 2016. National parks in the eastern United States harbor important older forest structure compared with matrix forests. Ecosphere 7(7):e01404. 10.1002/ecs2.1404

Miller, K.M., S.J. Perles, J.P. Schmit, E.R. Matthews, M.R. Marshall. 2023. Overabundant deer and invasive plants drive widespread regeneration debt in eastern United States national parks. Ecological Applications. 2023;33:e2837. https://onlinelibrary.wiley.com/r/eap

Potter, K.M and Riitters, K. 2022. A National Multi-Scale Assessment of Regeneration Deficit as an Indicator of Potential Risk of Forest Genetic Variation Loss. Forests 2022, 13, 19. https://doi.org/10.3390/f13010019.

Potter, K.M., K.H. Riitters, B.V. Iannone III, Q. Guo and S. Fei. 2024. Forest plant invasions in the eastern United States: evidence of invasion debt in the wildland‑urban interface. Landsc Ecol (2024) 39:207 https://doi.org/10.1007/s10980-024-01985-y

Potter, K.M., B.V. Iannone III, K.H. Riitters, Q. Guo, K. Pandit, C.M. Oswalt. 2026a. US Forests are Increasingly Invaded by Problematic Non-Native Plants. Forest Ecology and Management 599 (2026) 123281

Potter, K.M., Q. Guo, F.H. Koch, S. Lim-Hing, E.R. Matthews, and K. Pandit. 2026b. U.S. National Forests Are More Diverse, Denser and Less Invaded than Neighboring Forests. Forests 2026 17

Reichard, S.H. and P. White. 2001. Horticulture as a Pathway of Invasive Plant Introductions in the United States. BioScience 103. Vol. 51 No. 2. February 2021.

Riitters, K., K. Potter, B.V. Iannone III, C. Oswalt, S. Fei, Q. Guo. 2017. Landscape correlates of forest plant invasions: A high-resolution analysis across the eastern United States. Diversity and Distributions. DOI: 10.1111/ddi.12680

Tallamy, D.W. and K.J. Shropshire. 2009. Ranking Lepidopteran Use of Native Versus Introduced Plants

Conservation Biology, Volume 23, No. 4, 941–947 2009 Society for Conservation Biology

DOI: 10.1111/j.1523-1739.2009.01202.x

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
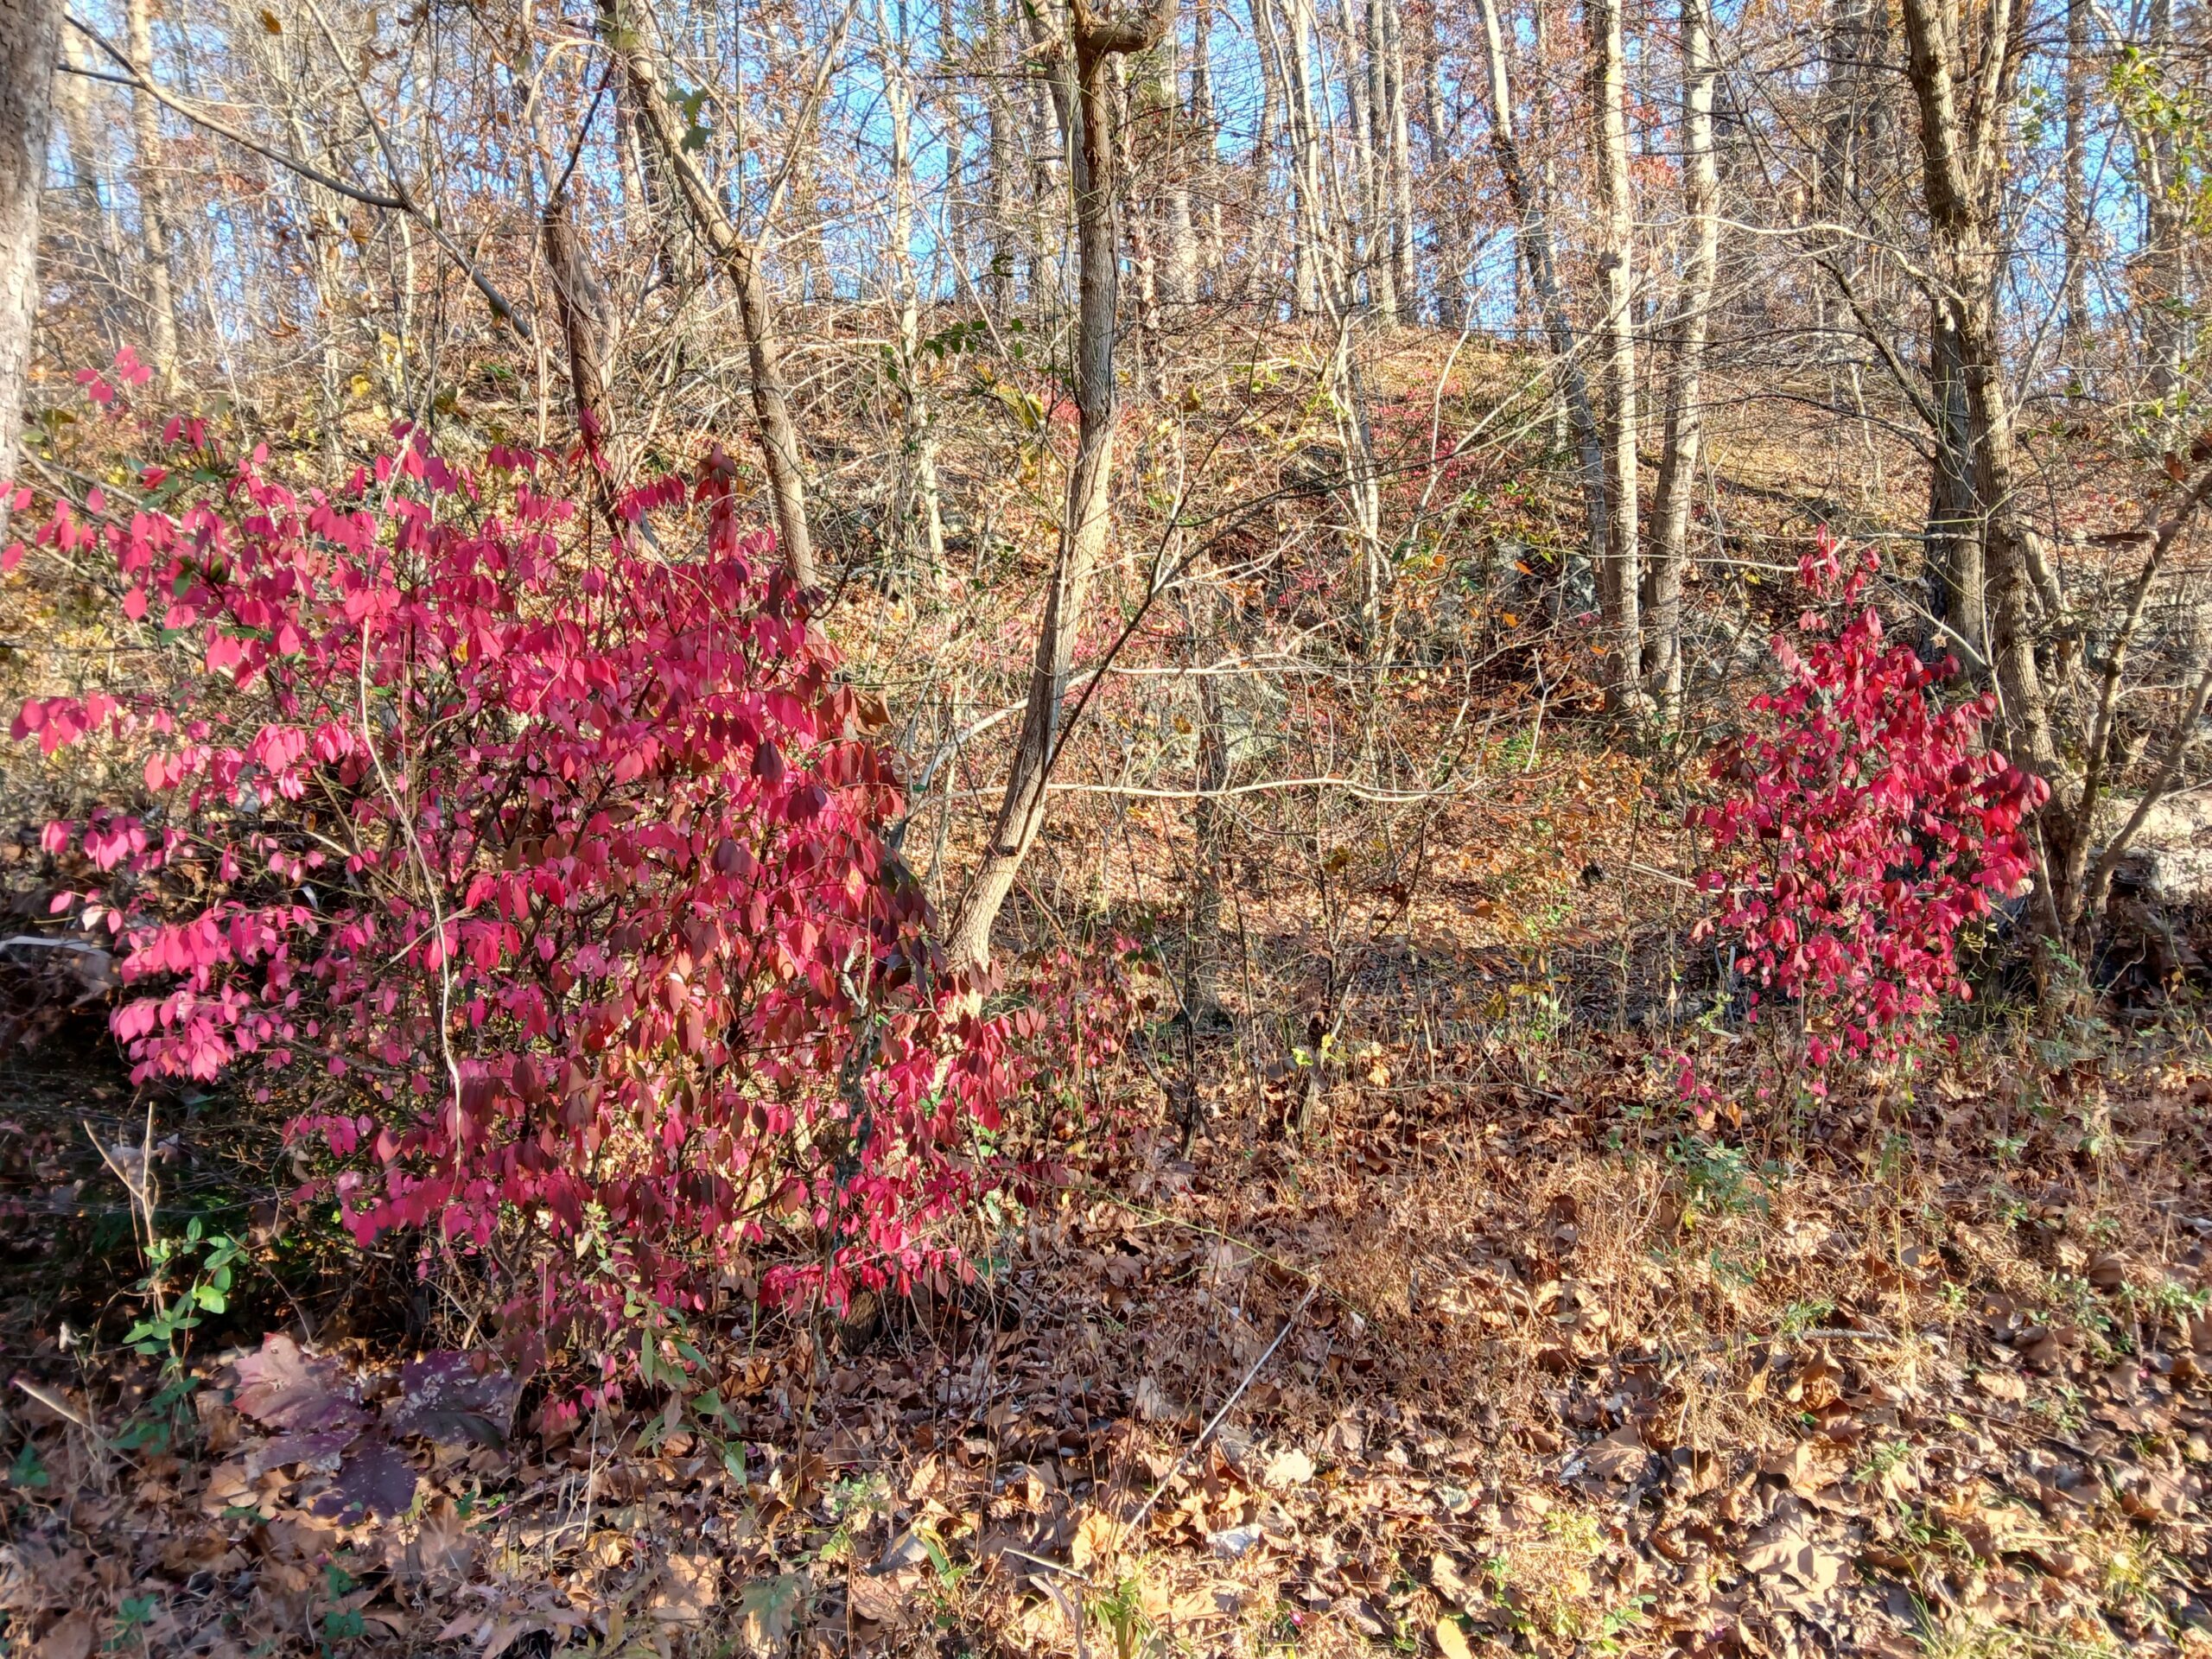
https://fadingforests.org

Invasive species on the African Continent

We are beginning to get more information about invasive species on the African continent.

a flyer naming principal invasive ornamental plants in Kruger National Park

In several countries, the focus has been on threats to agriculture. Previous blog about horizon-scanning in Ghana. In Zimbabwe, N. Mudada and colleagues (2026; full citation and the end of this blog) found alarming, if not surprising, levels of risk to food production from introduced invasive plants. They investigated 1,668 human-aided transboundary plant introductions at 14 ports of entry and non-official crossing points over the course of four years.

They estimate that the 20,000 trucks that transported maize into the country over the four years carried over 20,700 metric tons of weed seeds and rubbish! They recorded detections of 11 species in eight orders. The pathways are familiar. As noted, several weeds were contaminants of grain shipments; Convolvulus arvensis in wheat for human consumption, Helianthus annus and Datura stramonium in maize for animal feed. Adenium obesum and Vitex agnus-castus were being smuggled for planting as flowers and ornamentals. (Vitex agnus-castus was also smuggled in passenger baggage for its medicinal properties). Several Lemna species (an aquatic plant) were also smuggled for planting as animal feeds.

In some cases, the focus is the threat to native ecosystems. I posted a blog the about threat of an introduced pathogen to trees in the remnant rain forests of Madagascar.

South Africa still has the lead in addressing invasive species. Regarding invasive plants specifically, the country has the benefit of more than 150 years of botanizing. The richness of the region’s flora is globally recognized. South Africa also has a long history of studying and managing invasive species, especially plants.

South African scientists and colleagues in Botswana, Eswatini, Lesotho, and Namibia have published four editions of the Flora of the Southern Africa region since 1984. In 2006, the PRECIS database of the South African National Biological Diversity Institute (SANBI) was combined with the Tropical African Plant Checklist published by the Conservatory and Botanical Garden of Geneva to create the African Plant Checklist and Database Project. It is continually updated. This is the first continental flora checklist for Africa; it fulfils countries’ obligations under the Convention on Biological Diversity’s Global Strategy for Plant Conservation.

For South Africa specifically, scientists have produced a national plant checklist that is updated annually.

The 2025 Checklist reports that 21,539 plant species are extant outside cultivation in the country; these comprise 20,204 indigenous species and 1,329 naturalized species. Thus, 6% of the total flora is non-indigenous. Of these, 649 (48.8% of the non-indigenous species, 3% of all plants) of them are invasive.

[Naturalized species are defined as species whose documented natural range does not include South Africa, but have overcome a biogeographic barrier and now sustain self-replacing populations for two or more life cycles or over a given period of time in the country. These populations are maintained without direct intervention by people, or despite human intervention. Invasive species meet the above definition plus produce reproductive offspring, often in large #s at considerable distances from the parent and/or site of introduction, and have the potential to spread over long distances.]

Since the previous checklist was published in 2006, botanists have identified 1,048 additional species – a 4.9% increase. Eighty-two percent of the newly identified species (865 species) are “naturalized”. Specifically, 414 new species are categorized as naturalized (a 31.1% increase), and 451 new species are classified as invasive (a whopping 69.5% increase). Le Roux and Klopper attribute these steep increases to active botanizing by SANBI’s Invasive Species Programme (begun in 2008), and the Southern African Plant Invaders Atlas Project (begun in 2010).

Of the 384 plant families present in South Africa, 350 contain at least some indigenous species. Thirty-four families contain only naturalized species. Among the 2,189 plant genera present, 459 (21%) contain only species that are non-indigenous.

Three families stand out because of the particularly high numbers of naturalized species: Fabaceae (143 species; 11% of all naturalized species), Asteraceae (140 species; 10%), Poaceae (123 species; 9%). Two of these families — Asteraceae and Fabaceae — are also the largest families among native South African plants. The third, grasses (Poaceae), ranks seventh in the list of most specious families indigenous to South Africa. The next group of families with high numbers of naturalized species has less than half as many invasive species: Myrtacae (55), Amaranthacea (52), Solanaceae (48). None of these families ranked within the top 20 families of indigenous plant species.

The genera with the most naturalized species were Solanum, Euphorbia and Acacia (all 24 or 23 species).

Acacia cyclops; photo by David M. Richardson

South African scientists are also exploring how to balance conflicting goals and perspectives when an invasive plant species has economic or social value. The example chosen by Mbobo et al. (2025) is guava (Psidium guajava) – a nutritious and popular tropical fruit grown commercially in South Africa, but also invasive along roadsides, watercourses and forest margins. Invasions are especially common in eastern parts of country; large monocultures are found in KwaZulu-Natal. Outbreaks have also been detected at five sites in Western Cape in riparian zones and at a hot spring. Mbobo et al. (2025) note that the microclimatic conditions at this last location differ from the broader conditions in the region – which are what most models would measure.

The scientists used models to predict where guava might invade – especially in large monocultures – and compared those areas to where the tree can be grown in cultivation with human inputs, e.g., irrigation. They then assessed whether six regulatory approaches would avoid restricting guava farming in areas at minimal or low risk while still protecting vulnerable locations. They also considered the amount of information required to implement the approach and costs of acquiring the information; and level of likely public acceptance. Mbobo et al. (2025) laid out the trade-offs between continuing to regulate planting of the species at the provincial level vs. at the municipal level. Prohibiting planting of guava in provinces where it is recorded as invasive allows some plantings near natural forests and riparian areas that are highly susceptible to guava invasions. On the other hand, nearly half of the prohibited area is outside the known or likely at-risk area. The provinces do allow exceptions through a permit process. Adopting more geographically limited rules by regulating at the municipal level would enable a tighter link to geographic areas at highest risk. However, this approach does not address long-distance seed dispersal by animals. Furthermore, the very detailed regulations might confuse stakeholders and complicate enforcement. Also, the models lack sufficiently fine spatial resolutions to predict invasible areas so accurately. Finally, the reduction in regulated area is minimal (~ 14%), so the economic benefits are unlikely to outweigh the significantly higher administrative costs and risk of allowing guava invasions in new sites.

Guava fruit on tree; Roenashy via Wikimedia

Gildenhuys et al. (2026) analyzed the factors that drive which non-native plants establish where. They assessed the roles of temperature, precipitation, urbanization intensity, urban area, travel time, year of city’s establishment, and human population density in determining which plant species are present in 54 urban centers in Western Cape Province. The cities have significant differences in climate: Mediterranean in the far southwest, warm temperate in the southeast, and semi-arid towards the interior. The expectation was that these drivers and assembly processes are influential at more advanced invasion stages when the species have already overcome some barriers to dispersal, so are now found in reasonably suitable habitats.

Gildenhuys et al. (2026) found temperature and precipitation were most important in determining plant species’ presence. This was especially true at the boundary between arid and mesic climates. These strong environmental gradients are the same ones which have driven high differences in native species presence across the province. [See pamphlet describing invasive plants in Cape Town.] This finding supports the “Goldilocks hypothesis”: that non-native plant species assemblages are driven by the same abiotic variables as native species assemblages. While did not directly study the “Biome decides hypothesis” (the composition of non-native flora is mediated by the biotic effects of native flora and fauna), Gildenhuys et al. (2026) doubt its applicability here because native species’ presence has probably been greatly reduced by the effects of urbanization.

Urbanisation intensity itself ranked third as a factor. Its effect was strongest at low to medium urbanization intensities. Because urbanization creates novel habitats, such as, “hardscapes” of paved surfaces that resemble deserts, their non-native plant assemblages are dominated by similar, urban specialist, species. At lower urbanization intensities a greater variety of habitats is available. Gildenhuys et al. (2026) conclude that urbanization acts primarily as a driver of opportunistic habitats for species at later invasion stages rather than as a filter of species introduction.

An earlier study found a similar effect from road density (often associated w/ urbanization) as an explanation for where specific woody non-native species establish. They do concede that larger urban areas might experience greater propagule pressure.

Gildenhuys et al. (2026) note that recent globalization of the plant trade has probably changed the specis planted in urban centers. For example, cities in the Western Cape are increasingly replacing English oak (Quercus robur) with more disease-resistant oaks. The change might reflect greater environmental awareness and regulations issued under the National Environmental Management: Biodiversity Act 10 of 2004. In newly established urban centers, fewer invasive species are being planted — at least among trees.

SOURCES

Gildenhuys, C.P., L.J. Potgieter, C. Hui, D.M. Richardson. 2026. Drivers of compositional turnover of the NIS urban flora in the W Cape, South Africa. Urban Ecosystems (2026) 29:51 https://doi.org/10.1007/s11252-026-01919-3

Le Roux, M.M., R.R. Klopper. 2025. Taking stock of South Africa’s flora. South African Journal of Botany 184 (2025) 571-579

Mbobo, T., D.M. Richardson, A. Datta, K.T. Faulkner, J.R.U. 2025. Wilson. Spatially-Differentiated Reg of NIS Can Be Improved Using Spp Distribution Models: Psidium guajava in South Africa as a Case Study. Diversity and Distributions. 2025 31:e70102 https://doi.org/10.1111/ddi.70102

Mudada, N., J. Chitamba, E. Nyangani, C. Chapano, N. Mapope,and W. Ngezimana. 2026. Weeds associated with cross border traffic, their approach and infestation rates in Zimbabwe.  ISABB Journal of Food and Agricultural Sciences. Vol. 12(1) January-June 2026. DOI: 10.5897/ISABB-JFAS2025.0192

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
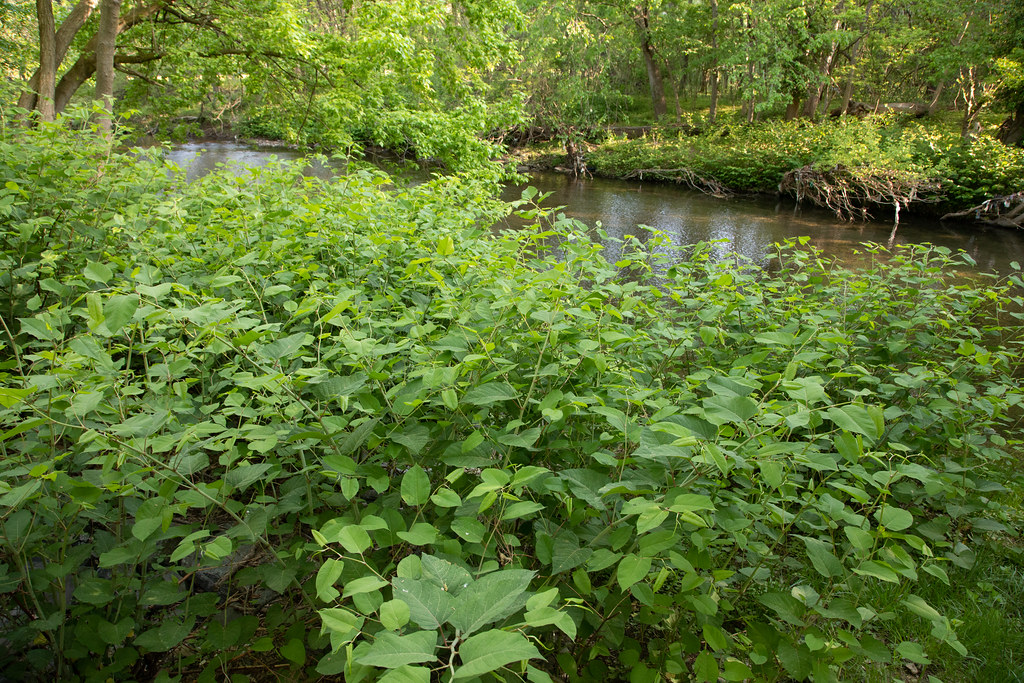
https://fadingforests.org

EAB infestation at 20 years: focus on green & white ash & white fringetree

dying ash in Shenandoah National Park; photo by F.T. Campbell

The emerald ash borer (Agrilus plannipennis; EAB) was detected in North America in 2002. So both U.S. and Canadians have been motivated to evaluate the probable trajectory of the primary hosts – the ash genus Fraxinus – in the face of the ongoing invasion. See Deschênes et al. 2026 and Wilson et al. 2025 – full citations at the end of this blog. Both studies focused on white (Fraxinus americana) and green ash (F. pennsylvanica); they say next to nothing about black ash (F. nigra). I regret this silence because of the unique ecology of black ash swamps. Neither addresses the threat to Oregon ash (F. latifolia) in the West.

The two assessments have similar findings: high mortality of larger trees (canopy and “recruit” size trees); abundant regeneration (seedling and saplings sizes) after an initial period; and uncertainty as to whether persisting EAB populations will kill the saplings before sufficient numbers grow into reproductive size.

There are two conspicuous differences. First, the American study does not consider the possible impact of biological control – although USDA APHIS has placed all its effort on this approach since January 2021. The Canadians report that self-sustaining populations of the wasps are now found across the northern U.S. and eastern Canada. In their study, conducted in Ontario, they detected only Tetrasticus planipennisi; it was parasitizing 16% of the EAB larvae in dissected stems. This wasp’s affinity for colder climates and short ovipositor – which limits it to parasitizing larvae inhabiting small stems – are portrayed as positive traits under these circumstances.

Second, the Canadians did not find “lingering” adult ash trees as have the Americans. These trees indicate the probability of finding workable levels of genetic resistance to the EAB. USDA Forest Service scientists are pursuing a breeding program.  While in south-central Michigan, where overstory ash mortality typically exceeded 80%, 46% of overstory ash and 82% of ash recruits were relatively healthy (Wilson et al. 2025), in Ontario none of 1,129 overstory ash trees survived beyond seven years after EAB detected. No trees exceeded 15 cm dbh (Deschênes et al. 2026).

ash resistance breeding trial at Holden Arboretum; photo courtesy of Jennifer Koch, USFS

Regeneration

As Deschênes et al. (2026) state, the future of ash stands depends on the complex of interactions among environmental conditions, management interventions, efficacy of natural enemies (natural or introduced), and life-history traits of the insect and its host. Coexistence might be possible if EAB larval densities remain sufficiently low to support survival of residual trees and successful seedling recruitment.

Larval densities in Ontario were said to be generally low, suggesting reduced carrying capacity in post-invasion forests, lower EAB fecundity, and higher EAB mortality in regenerating stems. Deschênes et al. (2026) note that in more northern areas colder temperatures are thought to slow larvae development. Perhaps these larvae might also be less vigorous, so they night disperse only over short distances. Still, there were sufficient EAB present after all the overstory trees had died to create 97% of the 298 galleries in regenerating ash stems (Deschênes et al. 2026). Furthermore, Wilson et al. (2025) say that EAB densities in infested trees in Michigan were similar to densities recorded during the initial invasion. This seems ominous to me – a solid foundation from which beetle populations could build up again as regenerating ash grow and provide more phloem for the insect to exploit.

Ash reproduce by both flowering/seeding and sprouting from the base. EAB predation is not the only complication. First, ash are dioecious so mature trees of both sexes must grow within a few hundred meters. Second, predation by the ash seed weevil (Lignyoodes helvolus) reduces seed supplies. Dense sedge mats can prevent germination (Wilson et al. 2025). Scientists generally believe that the soil seed bank is quickly exhausted, although Wilson et al. (2025) cite others’ conflicting findings. Neither article discusses predation by mammals, e.g., deer or rabbits. Wilson et al. (2025) mention attacks by beavers.

ash saplings felled by beavers; photo by F.T. Campbell

Wilson et al. (2025) did not study whether stump-sprouted ash were able to successfully recruit into the overstory. They do report that in one study in southeastern Michigan stump sprouts were the dominant form of green ash regeneration and about a quarter of these sprouts produced seeds at least once. Deschênes et al. (2026) found that on average 47% of regenerating stems at their Ontario research sites originated from stump sprouts.

EAB has been documented to attack and kill trees when the main stem is as small as 2.5 cm. While EAB probably prefer larger stems, Deschênes et al. (2026) suggest that stems become acceptable at the lower range of size required for seed production – 8–10 cm dbh. Reliable and abundant seed production doesn’t occur until white or green ash achieve > 20 cm dbh. At their Ontario sites, Deschênes et al. (2026) found that 42% of regenerating stems has been infested by EAB at least once; 14% had been attacked five or more times. They removed 74 EAB larvae from 28 stems; 49 (66%) were alive. Fifteen EAB (16% of current year galleries) had been parasitized — all by Tetrastichus planipennisi. They also observed numerous signs of defensive responses.

In Michigan, no ash recruits — living or dead – were found in plots in 28% of the cells. In the remaining 128 cells, an average of ~33% of ash recruits were infested by EAB, and ~21.4% of ash recruits dead. As is typical, white ash fared better than green ash. Recruit sized ash trees were twice as likely to die than to survive and mature into overstory size (Wilson et al. (2025).

In Ontario, as noted, all canopy ash had died. There were 119 live trees 5 – 10 cm dbh – a tenth as many “mature” ash as when EAB arrived, and all were smaller. There was abundant regeneration in most sites initially, but at the longest-infested sites in Essex County, regenerating ash stems were half as numerous as early after the transition (Deschênes et al. 2026).

The Canadians found it encouraging that some of the regenerating stems were vigorous despite containing EAB gallery densities greater than 20 larvae·m?2 of phloem. They did not know the mechanisms underlying survival of these stems. Possible explanations ranged from the low EAB carrying capacity of smaller trees to stronger host defenses in regenerating stems to EAB mortality due to parasitism.

Wilson et al. (2025) note that despite more than 20 years of EAB presence, densities of ash recruits, saplings, and seedlings were high relative to other species. However, they remind us, ~ one-third of the live ash recruits were infested so their survival into reproductive size was uncertain. The high mortality of overstory ash results in loss of seed resources, greater sun exposure, and cascading consequences for forest composition and function. In upland sites, cells with low ash basal area favored Quercus rubra and Tilia americana. They conclude that changes to forest composition is probably site specific — largely depend on what tree species are already present.

Despite the challenges described above, the Canadian scientists also believe that these findings demonstrate that ash has a capacity for long-term regeneration (Deschênes et al. 2026).

Changing Species Composition in the U.S.  (Wilson et al. 2025)

Canopy gaps caused by ash mortality have largely been filled by lateral ingrowth of species already there — American elm (Ulmus americana), black cherry (Prunus serotina), and northern red oak (Quercus rubra). The regeneration strata (saplings and seedlings) is dominated by Fraxinus (white outnumbering green when differentiated), maples (Acer rubrum, A. saccharum), black cherry, Crataegus species and Carya ovata. Elms are consistently among most common non-ash taxa among overstory, recruit, sapling and seedling strata. At some Ohio sites there was also increased abundance of non-native tree and shrub seedlings. This is not surprising since invasive plants are widespread in the forests of Ohio and other eastern states. A decade ago 93% of Forest Inventory and Analysis (FIA) plots in Ohio had at least one of 50 invasive plant species.

In another paragraph they mention Tilia americana as one of the important species in these forests.

Situation in Canada (Deschênes et al. 2026)

Deschênes et al. (2026) express concern that the death of nearly all canopy-level trees will substantially reduce ash’ ability to fulfill its ecological roles in these ecosystems. Still, ash regeneration is persisting for decades following overstory mortality. The taxon’s continued presence is driven largely by strong sprouting, which has been observed in several locations in Ontario. In some areas, low EAB infestation rates and evidence that regenerating stems can withstand multiple infestations raises hope that some might reach maturity and produce seeds. This scenario would be similar to that of elms, in which surviving trees contribute to ongoing regeneration and might eventually facilitate development of some level of resistance to the invasive fungus. A second possibility is that ash’ high sprouting capacity might point to a scenario similar to that of American chestnut. This species has persisted for a century primarily as sprouting shrubs — although they rarely reach reproductive maturity.

white fringetree; photo by Ryan Somma via Wikimedia

White Fringetree

Scientists also reviewed the status of a secondary host of EAB in North America, white fringetree (Chionanthus virginicus). Earlier studies of this host-pest relationship had been conducted on ornamental plantings where the trees tend to be scattered across open lawns and actively managed – including protection from pests. The Cipollinis (see full citation at the end of this blog) believe they might be better able to ward of EAB attack than are wild, unmanaged trees in forests that must compete for resources. They wanted to assess the current status and likely trajectory of the tree species in the wild.

To do so they revisited a wild population of the tree in southern Ohio previously assessed 10 years earlier. White fringetree is a small multi-stemmed tree native to the southeastern U.S. It is widely planted as an ornamental in across the east. In Ohio, white fringetree grows wild in only a few southern counties, in small populations or as widely scattered individuals. The species is classified as “Potentially Threatened” at the state level.

In 2015, 30% of the white fringetrees at the site were infested. These trees had signs of stress but none had died. EAB larvae grow more slowly on fringetree than on North American ash species. Meanwhile, all mature white ash trees at the site had been killed by EAB. Smaller white ash trees more comparable in size to the white fringetrees had attack rates and impacts comparable to those on the fringetrees.

In their new study, the Cipollinis found that nine of 31 trees tagged in 2015 (29%) had died; 22 (71%) were alive. Of those 22 living trees, 12 (55%) stayed the same or improved slightly over the five-year period; 10 (45%) declined. Five of these 22 living trees (23%) had evidence of current infestation. Trees that had died had a higher incidence of old EAB galleries, adult exit holes, and woodpecker activity. This is interpreted as demonstrating that EAB must cause extensive damage to kill fringetrees.

In summary, fringetrees in a wild unmanaged population continued to be attacked by EAB over 10 years and suffered higher attack rates and more significant impacts than those previously observed in managed pops. The Cipollinis conclude that trees large enough to attract EAB oviposition will continue to decline in health and be killed as long as beetles are present. They expect that wild white fringetrees might meet the same fate as ash trees, but over longer time scales. 

At the same time, this delay in complete mortality might create a refugium for remnant populations of EAB after most ash have been killed. This status would be exacerbated if it turns out that the biocontrol agents cannot find their target — EAB — in the alternative host. The Cipollinis found lower parasitism rates by Tetrastichus planipennisi in fringetrees, although this was not true for the egg parasite Oobius agrili and two Spathius larval parasites.

Whitebark fringetree populations can produce few adult EAB because the trees are small and contain low amounts of phloem. Still, as young trees grow into vulnerable sizes they might help sustain the EAB population – as young ash trees in the area appear to do.

While caution is appropriate in interpreting findings from a study of a single population, the Cipollinis argue that this population has been studied intensively: assessed six times over 10 years, beginning at the start of the EAB infestation. Therefore they think their analysis provides useful informative regarding the long-term impacts of EAB on fringetree.

They concede that larger populations in areas deep within the tree’s native range might experience different dynamics and impacts. So far, however, observations in Chattahoochee National Forest in Georgia and at Great Falls Park on the Maryland-Virginia border generally support their finding that wild fringetrees in natural landscapes will suffer higher attack rates and be more severely impacted by EAB than trees in managed landscapes.

Finally, the Cipollinis fear that a close relative, pygmy fringetree, Chionanthus pygmaeus, is at particularly high risk because it is endemic to only a few counties in the sandhills of central Florida. The species is already classified as endangered by both the state and the federal governments. The pygmy fringetree is smaller than white fringetree, so its size might help it escape attack. However, adults achieve sizes comparable to that of fringetree in some cases. So when EAB reaches Florida, the specie appears to be highly vulnerable.

SOURCES

Cipollini, D. and K. Cipollini. 2026  The Fate of a Wild White Fringetree (Chionanthus virginicus) Population in Ohio 10 Years After Invasion by Emerald Ash Borer (Agrilus planipennis) Forests 2026, 17, 712

Deschênes, É., C.J.K. MacQuarrie, L. Scott, C. Zimmerman, and I. Aubin. 2026. Ash population dynamics after two decades of emerald ash borer infestations in Canada. Canadian Journal of Forest Research. Can. J. For.Res. 56: 1–13 (2026) | dx.doi.org/10.1139/cjfr-2026-0075

Wilson, C.J, L. Labbate, T.R. Petrice, T.M. Poland, D.G. McCullough. 2025. Ongoing regeneration of ash and co-occurring species 20 years following invasion by emerald ash borer. Forest Ecology and Management 580 (2025) 122546


Posted by Faith Campbell

  We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

  For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

  Or
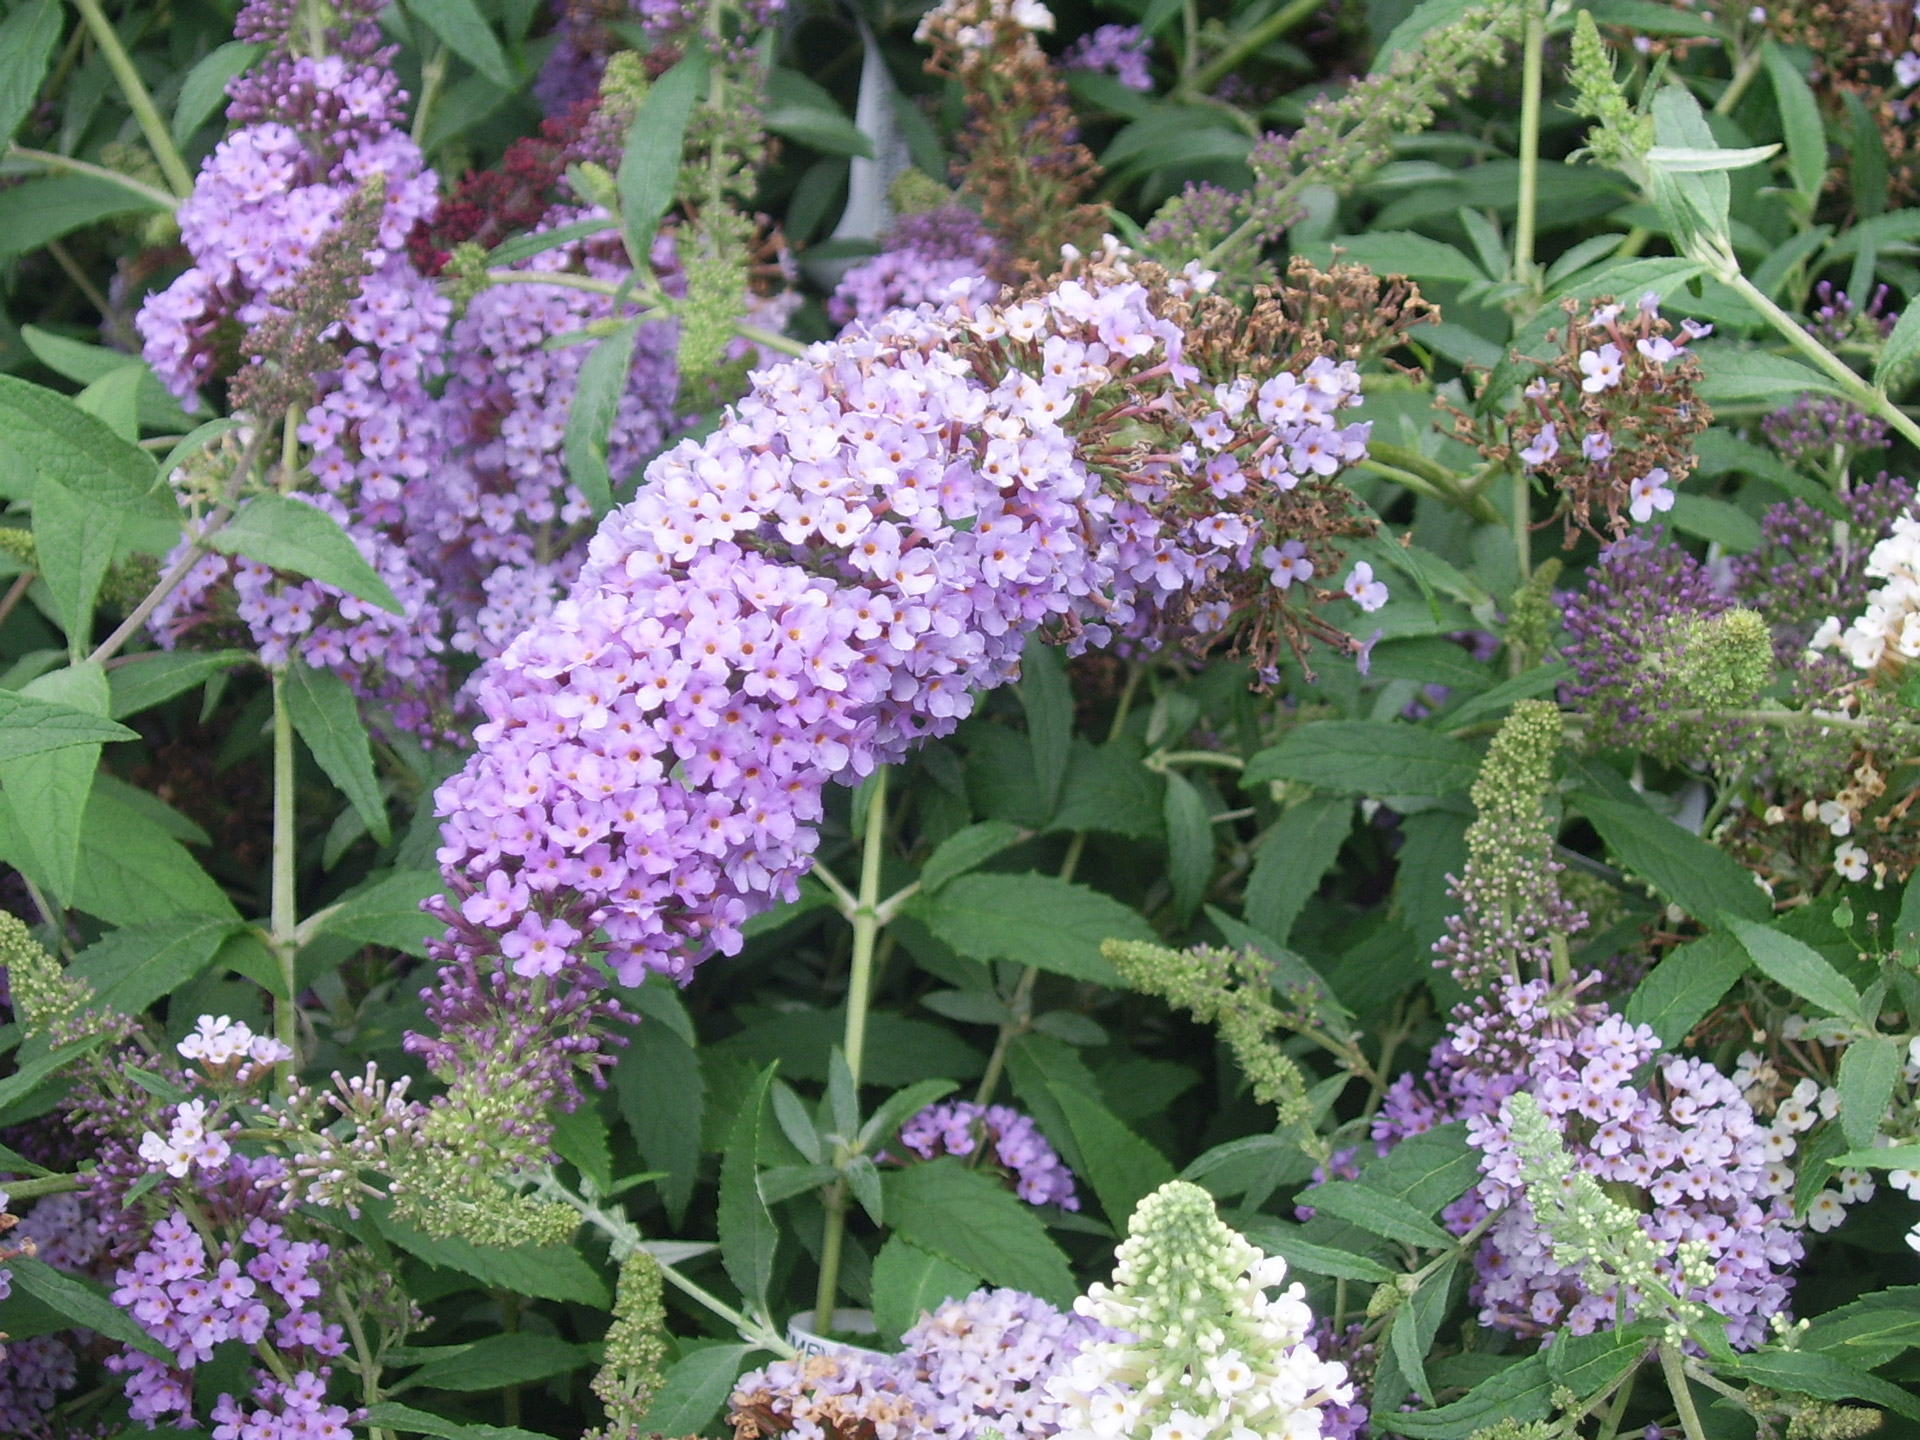
https://fadingforests.org