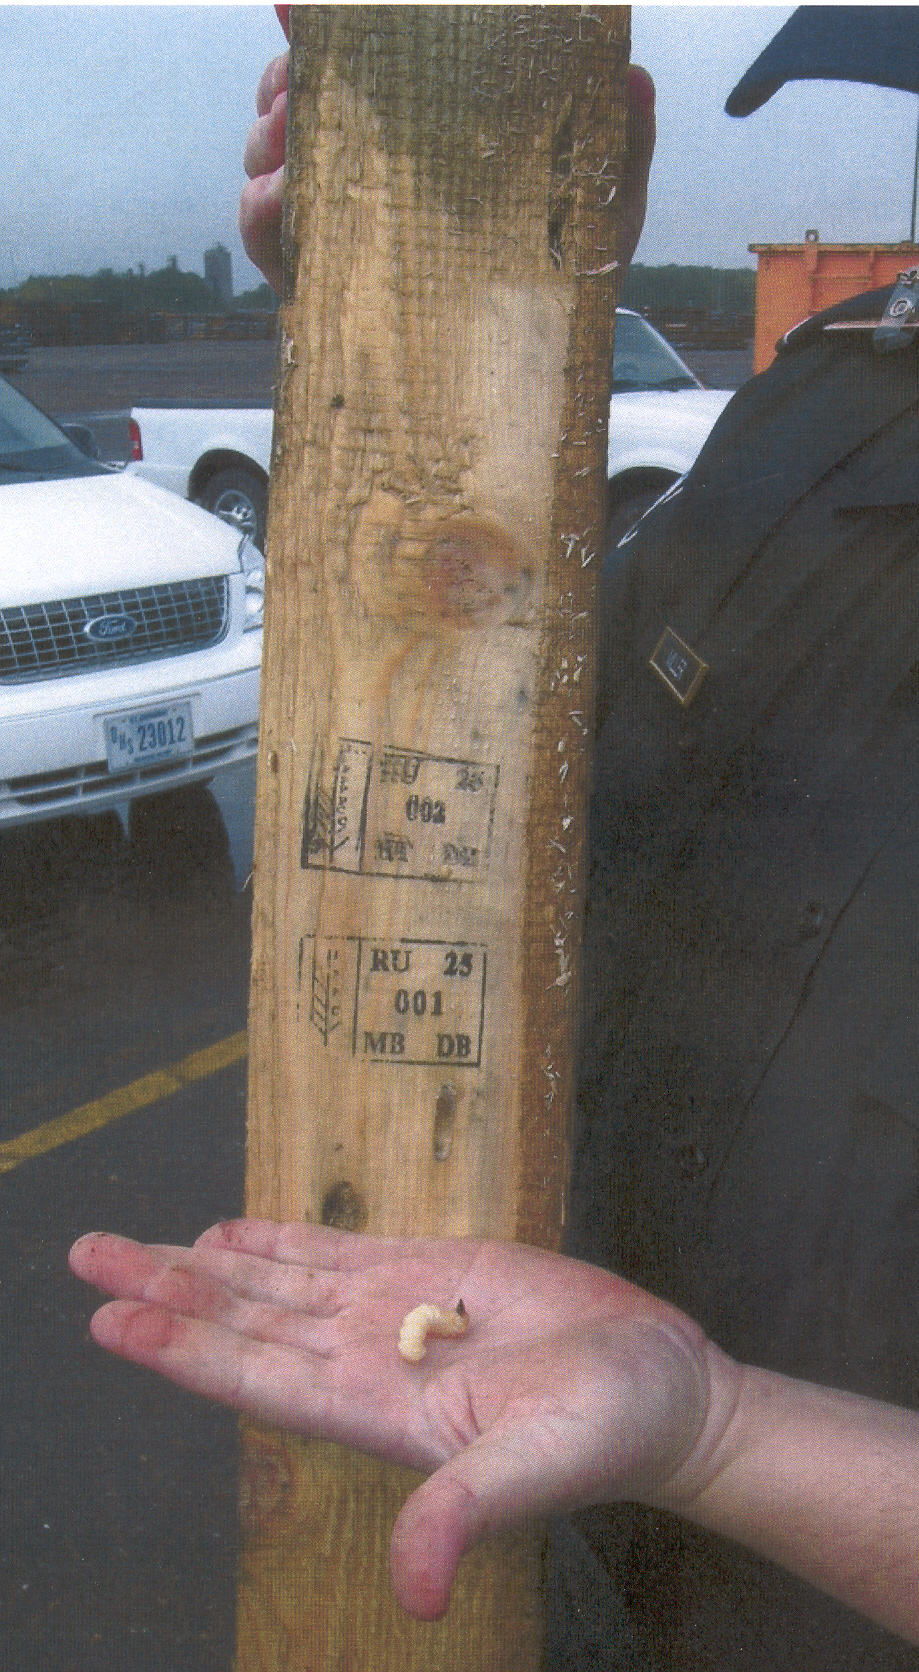
Twenty-four years ago the international community adopted ISPM#15 with the aim of reducing forest pest introductions via the wood used to make crates, pallets, and other forms of wood packaging (SWPM). Over that period questions have been raised about its efficacy. See the analyses by Haacket al. I have posted numerous blogs about wood packaging introductions, focused on the United States. To review these, on this website, scroll below the “Archives” to “Categories”, click on “wood packaging”.
Scientists continue to analyze data on wood borer introductions to explore patterns and evaluate the standard’s efficacy. Two recent articles focus on woodwasps in the Siricidae (Nardi et al. 2026) and ambrosia beetles in the Euwallacea complex (Lanschler et al. 2026). Full citations for both are at the end of this blog.
Sirex woodwasps
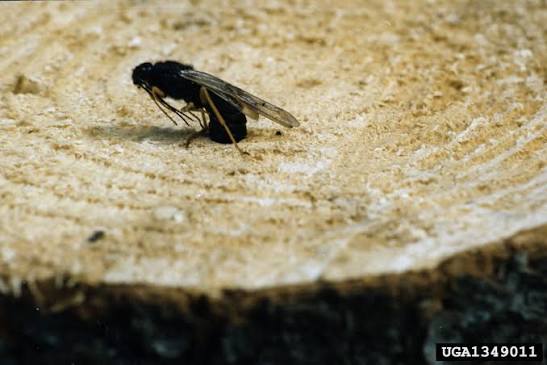
S. noctilio in Argentina; photo by Paula or Vicki Klasmer via Bugwood
A group of scientist led by D. Nardi surveyed woodwasp introductions to the United States, Canada, and New Zealand to determine historic and current patterns. They found that:
1) Nearly all Sirex woodwasps (84.2% – 97.6%) are transported in wood packaging.
2) While most introductions originated in the woodwasps’ native regions of Europe and Eastern Asia, accompanying high volumes of commodities imported from those regions, interceptions from the Southern Hemisphere have increased recently. Nardi et al. speculate that Asian countries might use softwoods (conifer species) less often for SWPM than do Europe and North America. Certainly the most infamous invasive wood borers from Asia are those that attack hardwoods, e.g., Asian longhorned beetle, emerald ash borer, invasive shothole borers.
3) Widespread adoption of ISPM#15 has significantly reduced interception, establishment, and damage associated with Siricids in the U.S., Canada, and New Zealand since 2002. However, continued detection of live Siricids in wood packaging demonstrates the need for strict enforcement of the standard’s provisions and potentially adoption of additional mitigation strategies.
4) Data collected by phytosanitary agencies of these importing countries is sometimes too limited to support needed analyses of trade patterns and risk.
U.S. phytosanitary agencies identified less than 10% of the intercepted woodwasps to the species level, whereas Canada identified 25% and New Zealand 75%. Identification of the intercepted woodwasp and its country of origin is critical for effective biosecurity. Nardi et al. (2026) express consternation that only 17.8% of interceptions were identified to species level. Even worse, U.S. phytosanitary officials identified less than 10% of the intercepted woodwasps to species. Canadian officials identified 25%, and New Zealand officials identified 75%. Yes, the taxonomy of the family is complex and in flux. And U.S. port staff must process orders of magnitude more interceptions of woodwasps than do either Canada or New Zealand. However, to understand which species are approaching American borders USDA APHIS (which performs the identifications) needs to provide specialized training and apply modern tools e.g., barcoding, molecular diagnostics. CBP and APHIS must also allow adequate time to process the detection before determining the fate of the shipment.
U.S. authorities also did not document the country of origin of 83% of shipments associated with Siricid-infested wood packaging intercepted. New Zealand authorities recorded the country of origin of 78% of intercepted shipments, Canadians of 90%.
Lack of information on sampling effort impedes exploitation of valuable info. Haack et al. (2014) discuss this obstacle in detail. Nardi et al. (2026) note that changing inspection and reporting priorities – especially when not explicitly described – hamper analysis of which factors explain variations in interception rates over time.
5) Interceptions of Siricids on wood packaging from regions outside the species’ native range have been increasing since the 1960s. Overall, 2.2% of the 504 interceptions named to species level were imported from countries to which they are not native. This included 12.3% of Sirex noctilio (from North America, the Neotropics, and Africa); 3.2% of Urocerusgigas (from North America and the Neotropics).
These secondary invasions are often from “bridgehead” populations in the Southern Hemisphere. Nardi et al. (2026) worry that such invasion bridgeheads established in trade hubs could speed up biological homogenization of their region.
6) Only a few of the more than 100 species in the family have established in novel regions although many additional species have frequently been intercepted in wood packaging by port inspectors. The species that have established are Sirex noctilio (introduced from Eurasia to North and South America, Australia, New Zealand, and South Africa); and two North American species: Urocerus albicornis (introduced to Europe and Asia) and Sirex obesus to South America. This pattern suggests that biological, environmental, or dispersal barriers interfere with establishment of other Sirex species even when they are transported to new regions.
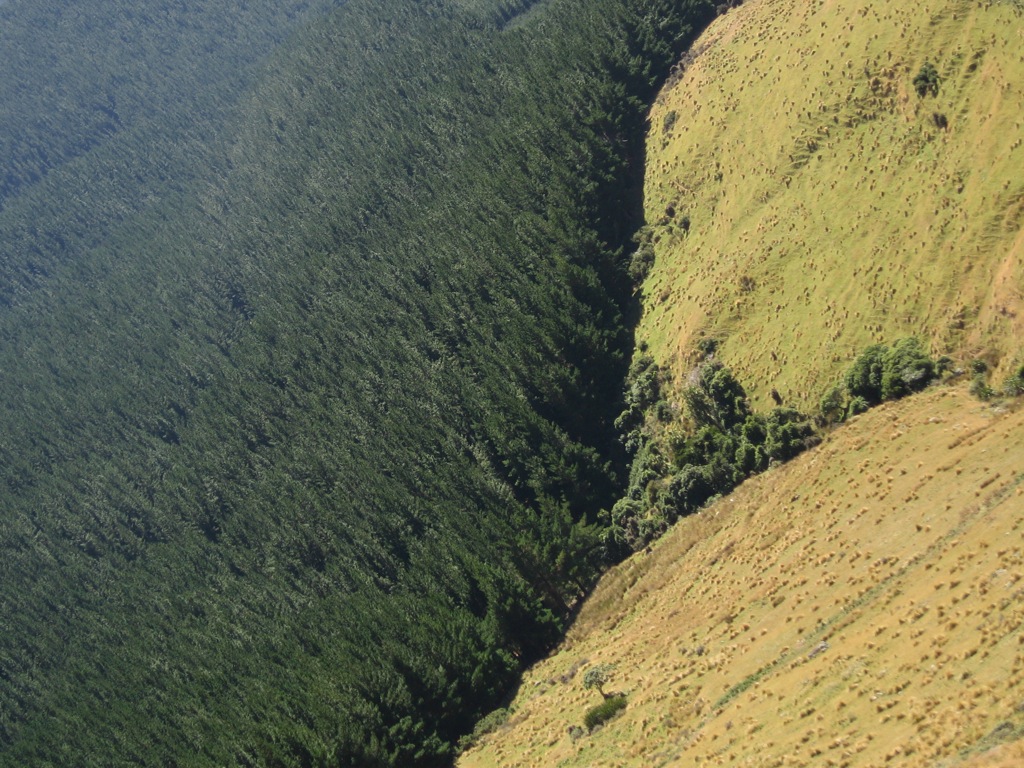
exotic pine plantation in New Zealand; photo by Jon Sullivan via Flickr
One example might be Sirex juvencus. Although it has been intercepted 215 times by one of the three countries, it has not established outside its native range. Nardi et al. (2026) note that the species prefers spruce (Picea spp.), which are much less commonly planted in Southern hemisphere plantations and around the Northen Hemisphere than the pines (Pinus spp.) that support establishment of S. noctilio and U. gigas.
The role of the associated fungi is another factor. Nardi et al. (2026) note that another woodwasp species, Xeris spectrum, has not established in New Zealand despite being intercepted often by that country’s phytosanitary officials and presence of suitable hosts. They note that is species does not transport the symbiotic fungi on its body as do other woodwasps. Instead it oviposits on trees already infested with Amylostereum fungus that was injected by an earlier invasive woodwasp. (A successful biological control program has reduced infestations of S. noctilio, so pine plantations are again widespread on the islands.)
Nardi et al. (2026) warn about several cryptic dangers. First, horizontal transfer of associated symbiont basidiomycete fungal species has been documented: Amylostereum fungal strains from European S. noctilio to American Urocerus species. Such transfers might increase the pathogenicity of formerly benign introductions. Second, scientists don’t yet understand the probable effects of climate change on insect and fungal species’ life cycles. They mention specifically the Asian species Sirex nitobei because its hosts are widespread Pinus species and it has been detected repeatedly, esp. on dunnage.
Nardi et al. (2026) suggest that officials should consider these ecological factors in assessing the risk of new introductions of specific species. I counter that the underlying rationale for adopting ISPM#15 was recognition that trying to manage individual species or countries of origin would not be effective. Instead, I advocate much more assertive enforcement of the standard.
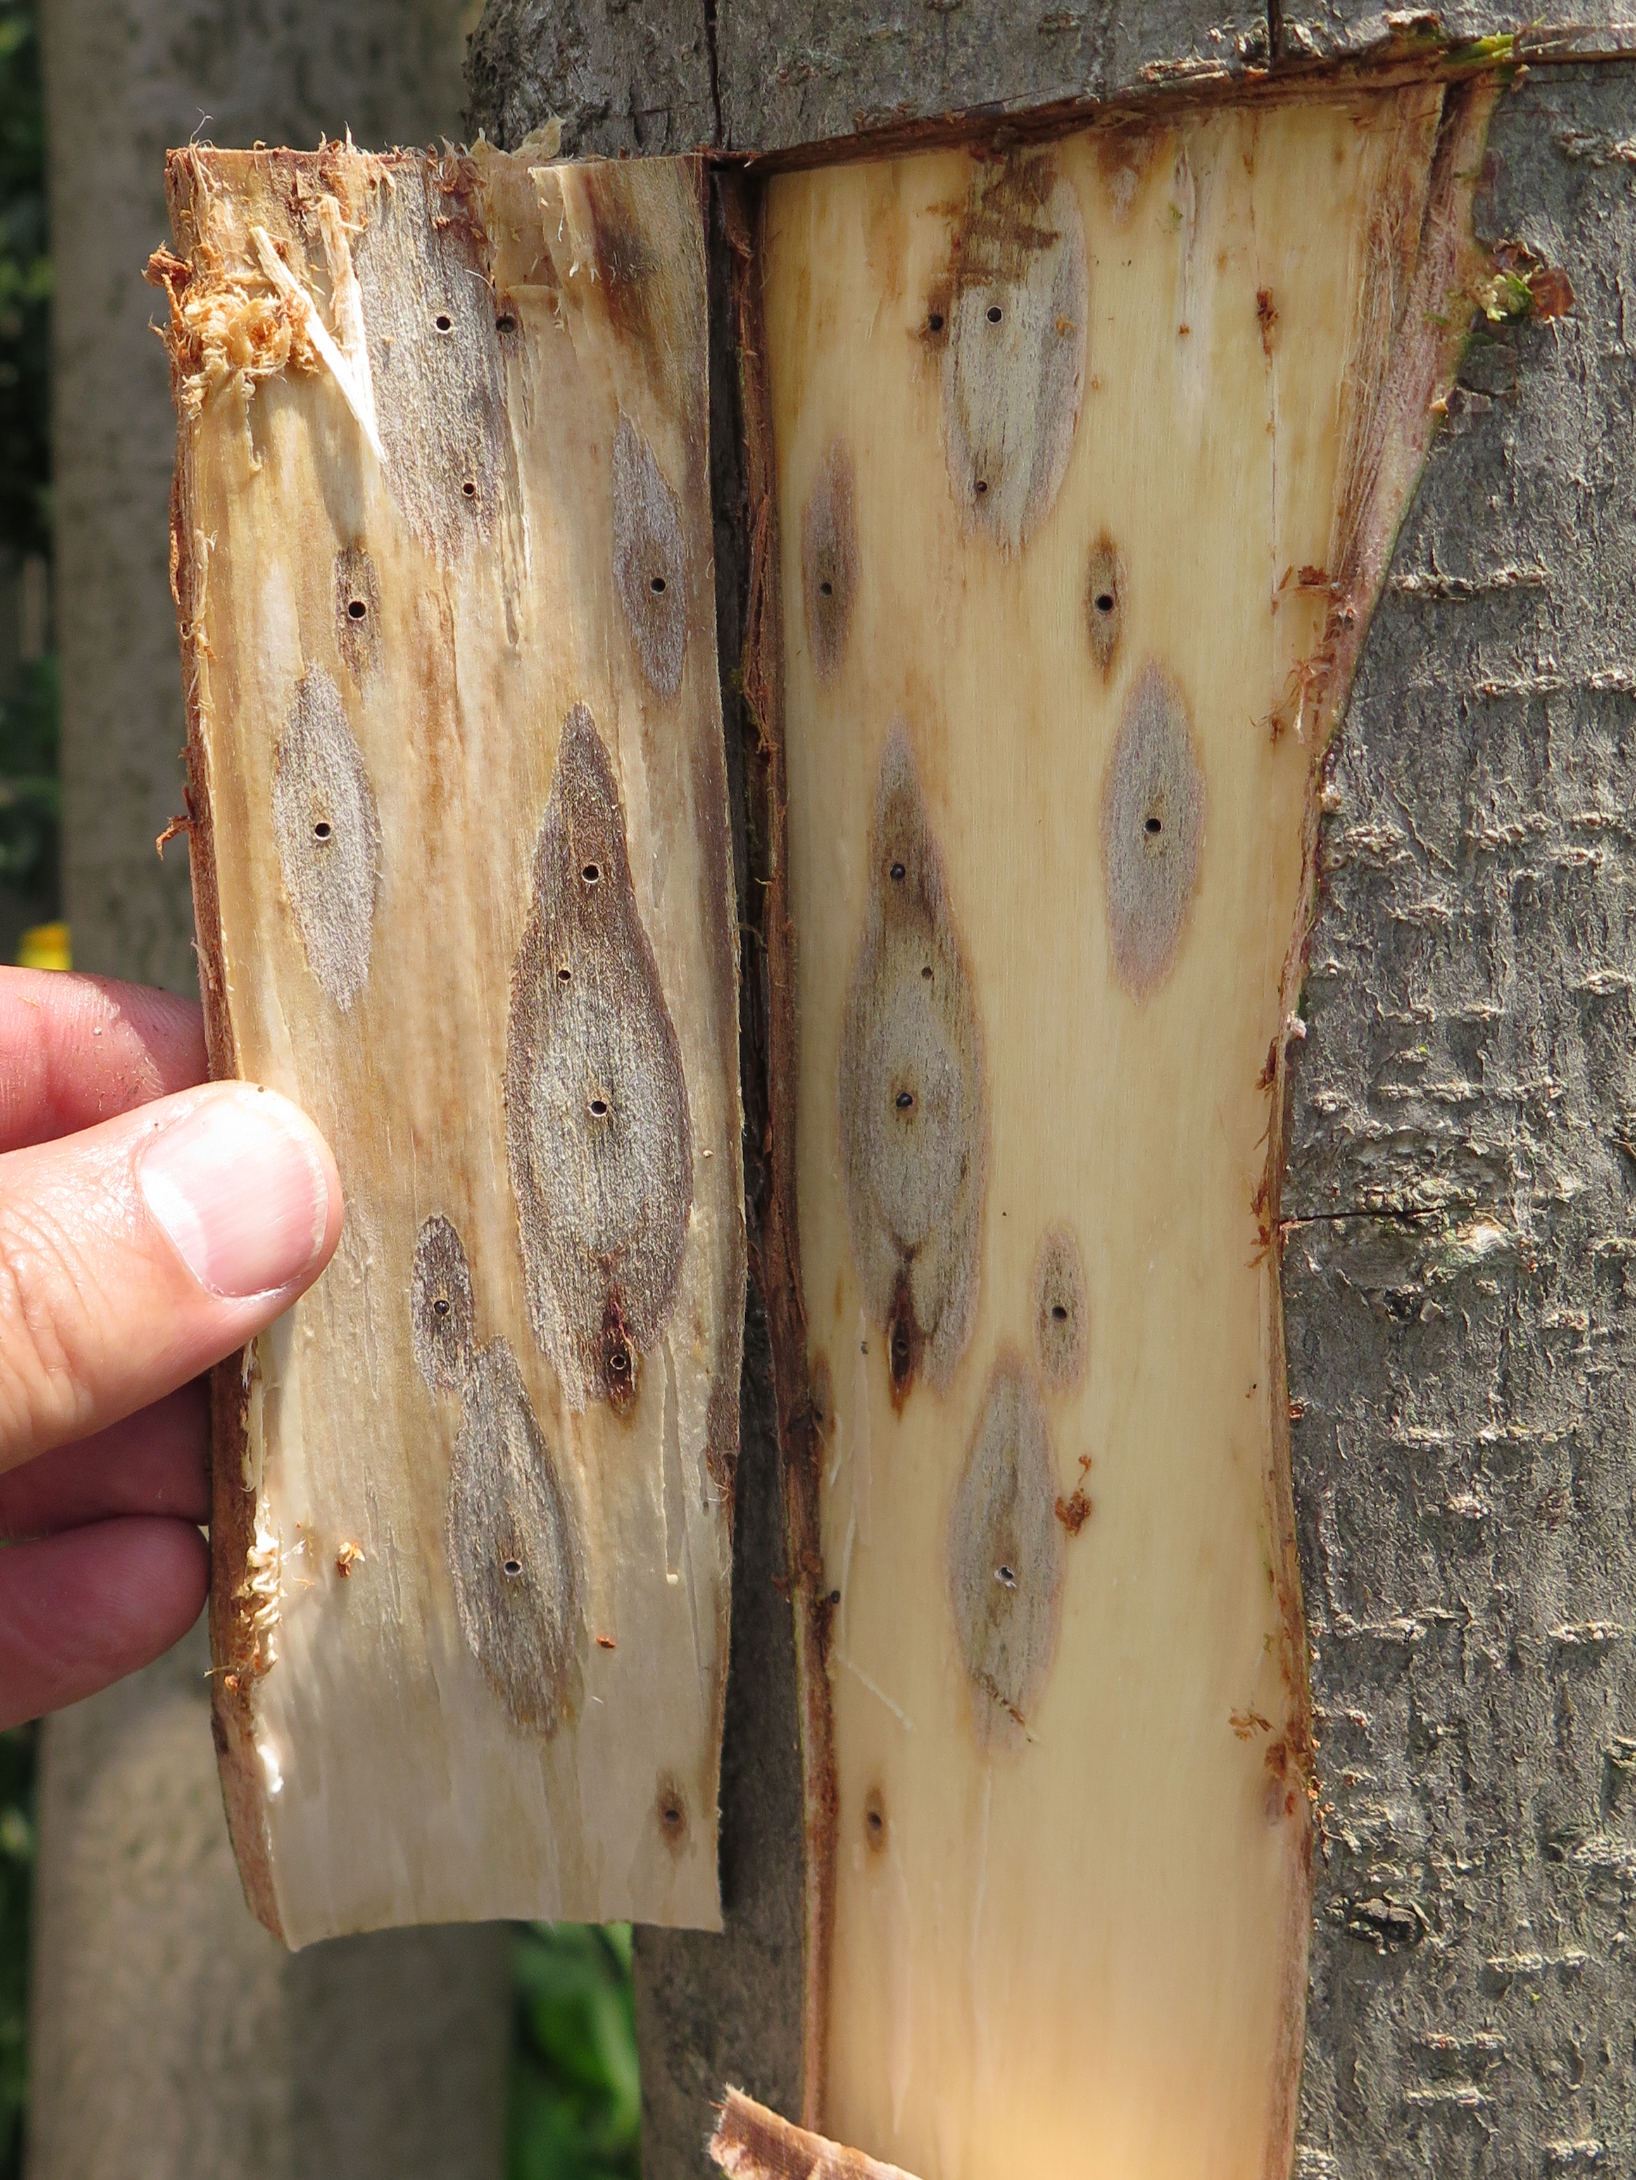
PSHB damage to Harepephyllum caffrum tree in South Africa; photo by Trudy Paap
Invasive shothole borers
Based on analysis on distribution of haplotypes, phylogenetic relationships and dates of first detections, Lantschner et al. (2026) identified seven independent introduction events of the polyphagous shot hole borer (PSHB) Euwallacea fornicatus: to the continental U.S., Hawai`i, South America, Central Europe, Spain, Türkiye, and South Africa. Most apparently originated directly from the species’ native range, although some evidence of likely secondary spread between already invaded regions. Several of these introductions – Israel (2009), South Africa (2016); Brazil (2020), Argentina and Australia (2021), Spain (2022), Uruguay (2023), and Türkiye (2024) – occurred despite stricter biosecurity measures, specifically ISPM#15.
The United States (California) experienced two additional invasions by Euwallaceae in the 2020s: by PSHB E. fornicatus (in San Jose) and a new species, E. interjectus. This makes a total of nine separate introductions.
Lantschner et al. (2026) suggest two opposite explanations for why so many introductions of this group of species from Asia have continued since ISPM#15 came into effect. Their suggestions are that either beetle populations in China, Taiwan, and/or Vietnam grew, thus increasing the pool of potential invaders/propagule pressure, or that increased international exports from these countries opened new commercial pathways. Certainly the latter has occurred. According to Google, exports from China rose from less than $500 billion in 2003 to ~ $4 trillion in 2025. Exports from Vietnam rose from ~$22 billion to $500 billion over the same period.
To be fair, most consider that the principal pathway for movement of species in the Euwallaceae complex is the trade in ornamental plants. In addition to the introductions listed above, E. fornicatus populations have been detected in greenhouses or botanical gardens in Italy, Germany, the Netherlands, and Poland. All have been reported as eradicated (Lantschner et al. 2026). I recently posted a blog discussing the widespread failure of the international phytosanitary system to stem introductions via this trade.
A second group of scientists (Dell, Xu, and Chi 2026) worry that E. fornicatus has spread especially rapidly in South Africa and South America. Already the outbreak of Fusasrium disease in South Africa is the largest the world: it is present in every province except Limpopo. The disease is recorded on 162 tree species, 78 of which are indigenous to the country (Townsend, Hill, Hurley and Roets 2025).
The introduced ranges – sometimes called bridgeheads – create conditions under which the pest can more easily spread further. Lantschner et al. (2026) suggest that the PSHB population established in southern California could spread into the American southeast, eastern Mexico, and parts of Central America. The population in South Africa might expand into other temperate and subtropical regions of Africa. Beetle populations established in Spain, Israel and Türkiye might spread across Mediterranean basin. Population in Western Australia could spread to eastern regions. They note that achieving some of these dispersals would require crossing substantial gaps of unsuitable habitat. They don’t mention that human transport has moved many populations of wood-boring beetles across unsuitable habitat! As I blogged earlier, officials in Sydney, Australia, determined that 47% of trees in the city are vulnerable to PSHB.
SOURCES
Carnegie AJ, Summerell BA, Trollip C, Tovar F, Smith DI and McDonald J (2026) Sentinel trees for early detection of non-native forest pests and pathogens in AU. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183
Dell, B., W. Xu, and N.M. Chi. 2026. Polyphagous Shot Hole Borer, a Global Threat to Forest Plantations, Green Infrastructure, and Biodiversity: Status, Challenges, and Solutions. Forests 2026, 17, 832
Lantschner, M.V., E. Ceriani-Nakamurakare, A.J. Johnson, A.I. Cognato, S.M. Smith, D.F. Gomez. 2026. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis (Coleoptera: Scolytinae), two global emerging pests. J Pest Sci 99, 100 (2026). https://doi.org/10.1007/s10340-026-02070-w
Nardi, D., K.E. Wagner, S.F. Ward, A.M. Liebhold, E.G. Brockerhoff, R.M. Turner, J.J. Riggins. 2026. Global movement of woodwasps (Hymenoptera: Siricidae) inferred from border interception records Biol Invasions (2026) 28:167 https://doi.org/10.1007/s10530-026-03881-9
Townsend, G., M. Hill, B.P. Hurley, and F. Roets. 2025. Escalating threat: increasing impact of the polyphagous shot hole borer beetle, Euwallacea fornicatus, in nearly all major South African forest types. Biol Invasions (2025) 27:88 https://doi.org/10.1007/s10530-025-03551-2
Posted by Faith Campbell
We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.
For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm
The international movement of plant material, particularly plants for planting, is widely acknowledged as a principal driver of the global eruption of forest health epidemics (Brasier, 2008; Turbelin et al., 2017; Tanney et al. 2025; Burgess and Wingfield 2026). The international plant health (or phytosanitary) community in 2012 adopted ISPM#36, with the goal of reducing pest and pathogen introductions on nursery stock. (“Plants for planting” is the regulatory term for this stock.) However, the top pages of the International Plant Protection Convention’s (IPPC) website do not mention either this issue or the IPPC’s response – this international standard!
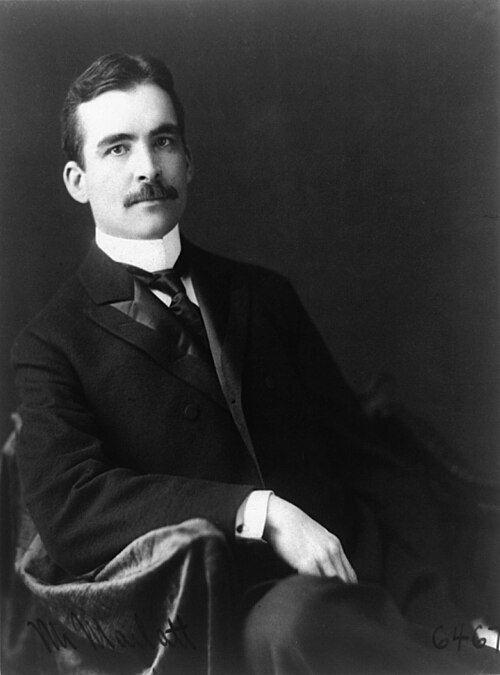
Charles L. Marlatt
Actually, awareness of this risk dates to the 19th Century, at least in Europe. USDA entomologist Charles Marlatt campaigned for the United States to impose phytosanitary rules beginning in 1911. He published a bulletin warning that the U.S. had become a “dumping ground” for contaminated nursery stock from Europe and urged the Congress to act. Marlatt is most famous for requiring destruction of diseased cherry trees sent as a gift by Japan. Liebhold and Griffin, in their summary of these events, do not comment on the fact that Marlatt acted without Congressional authority, although destruction of the cherry trees received permission from President Taft. Diplomatic exchanges resulted in Tokyo sending a new batch of pest-free cherries – their descendants grace the Tidal Basin and other parts of Washington, D.C. to this day. At Marlatt’s urging, and following realization of the damage caused by white pine blister rust, Congress adopted the Plant Protection Act in 1912.
This shows that it is possible to protect America’s flora while still enjoying imported plants. But this requires prompt and decisive action, well-prepared in advance, without the likelihood of legal challenges.
Pathogen and Pest Invasions Are Predictable Outcomes
Tanney et al. (2025) say it this way: “We trade not just in plants but also in phytobiomes.” [The phytobiome is the community of microorganisms living on and within a plant.] Burgess and Wingfield (2026) pronounce that invasions are not anomalies but rather predictable outcomes of global commerce interacting with ecological susceptibility. The global nursery trade creates extensive networks that enable the continuous exchange of live plant material across continents. Unlike many others, Burgess and Wingfield (2026) focus not on ornamental horticulture but the repeated occurrence of devastating outbreaks in Eucalyptus and Pinus plantations across the Southern Hemisphere.
Despite a century of efforts to curtail harmful introductions and 70 years after formation of the IPPC, devastating arthropods and disease pathogens continue to be introduced.
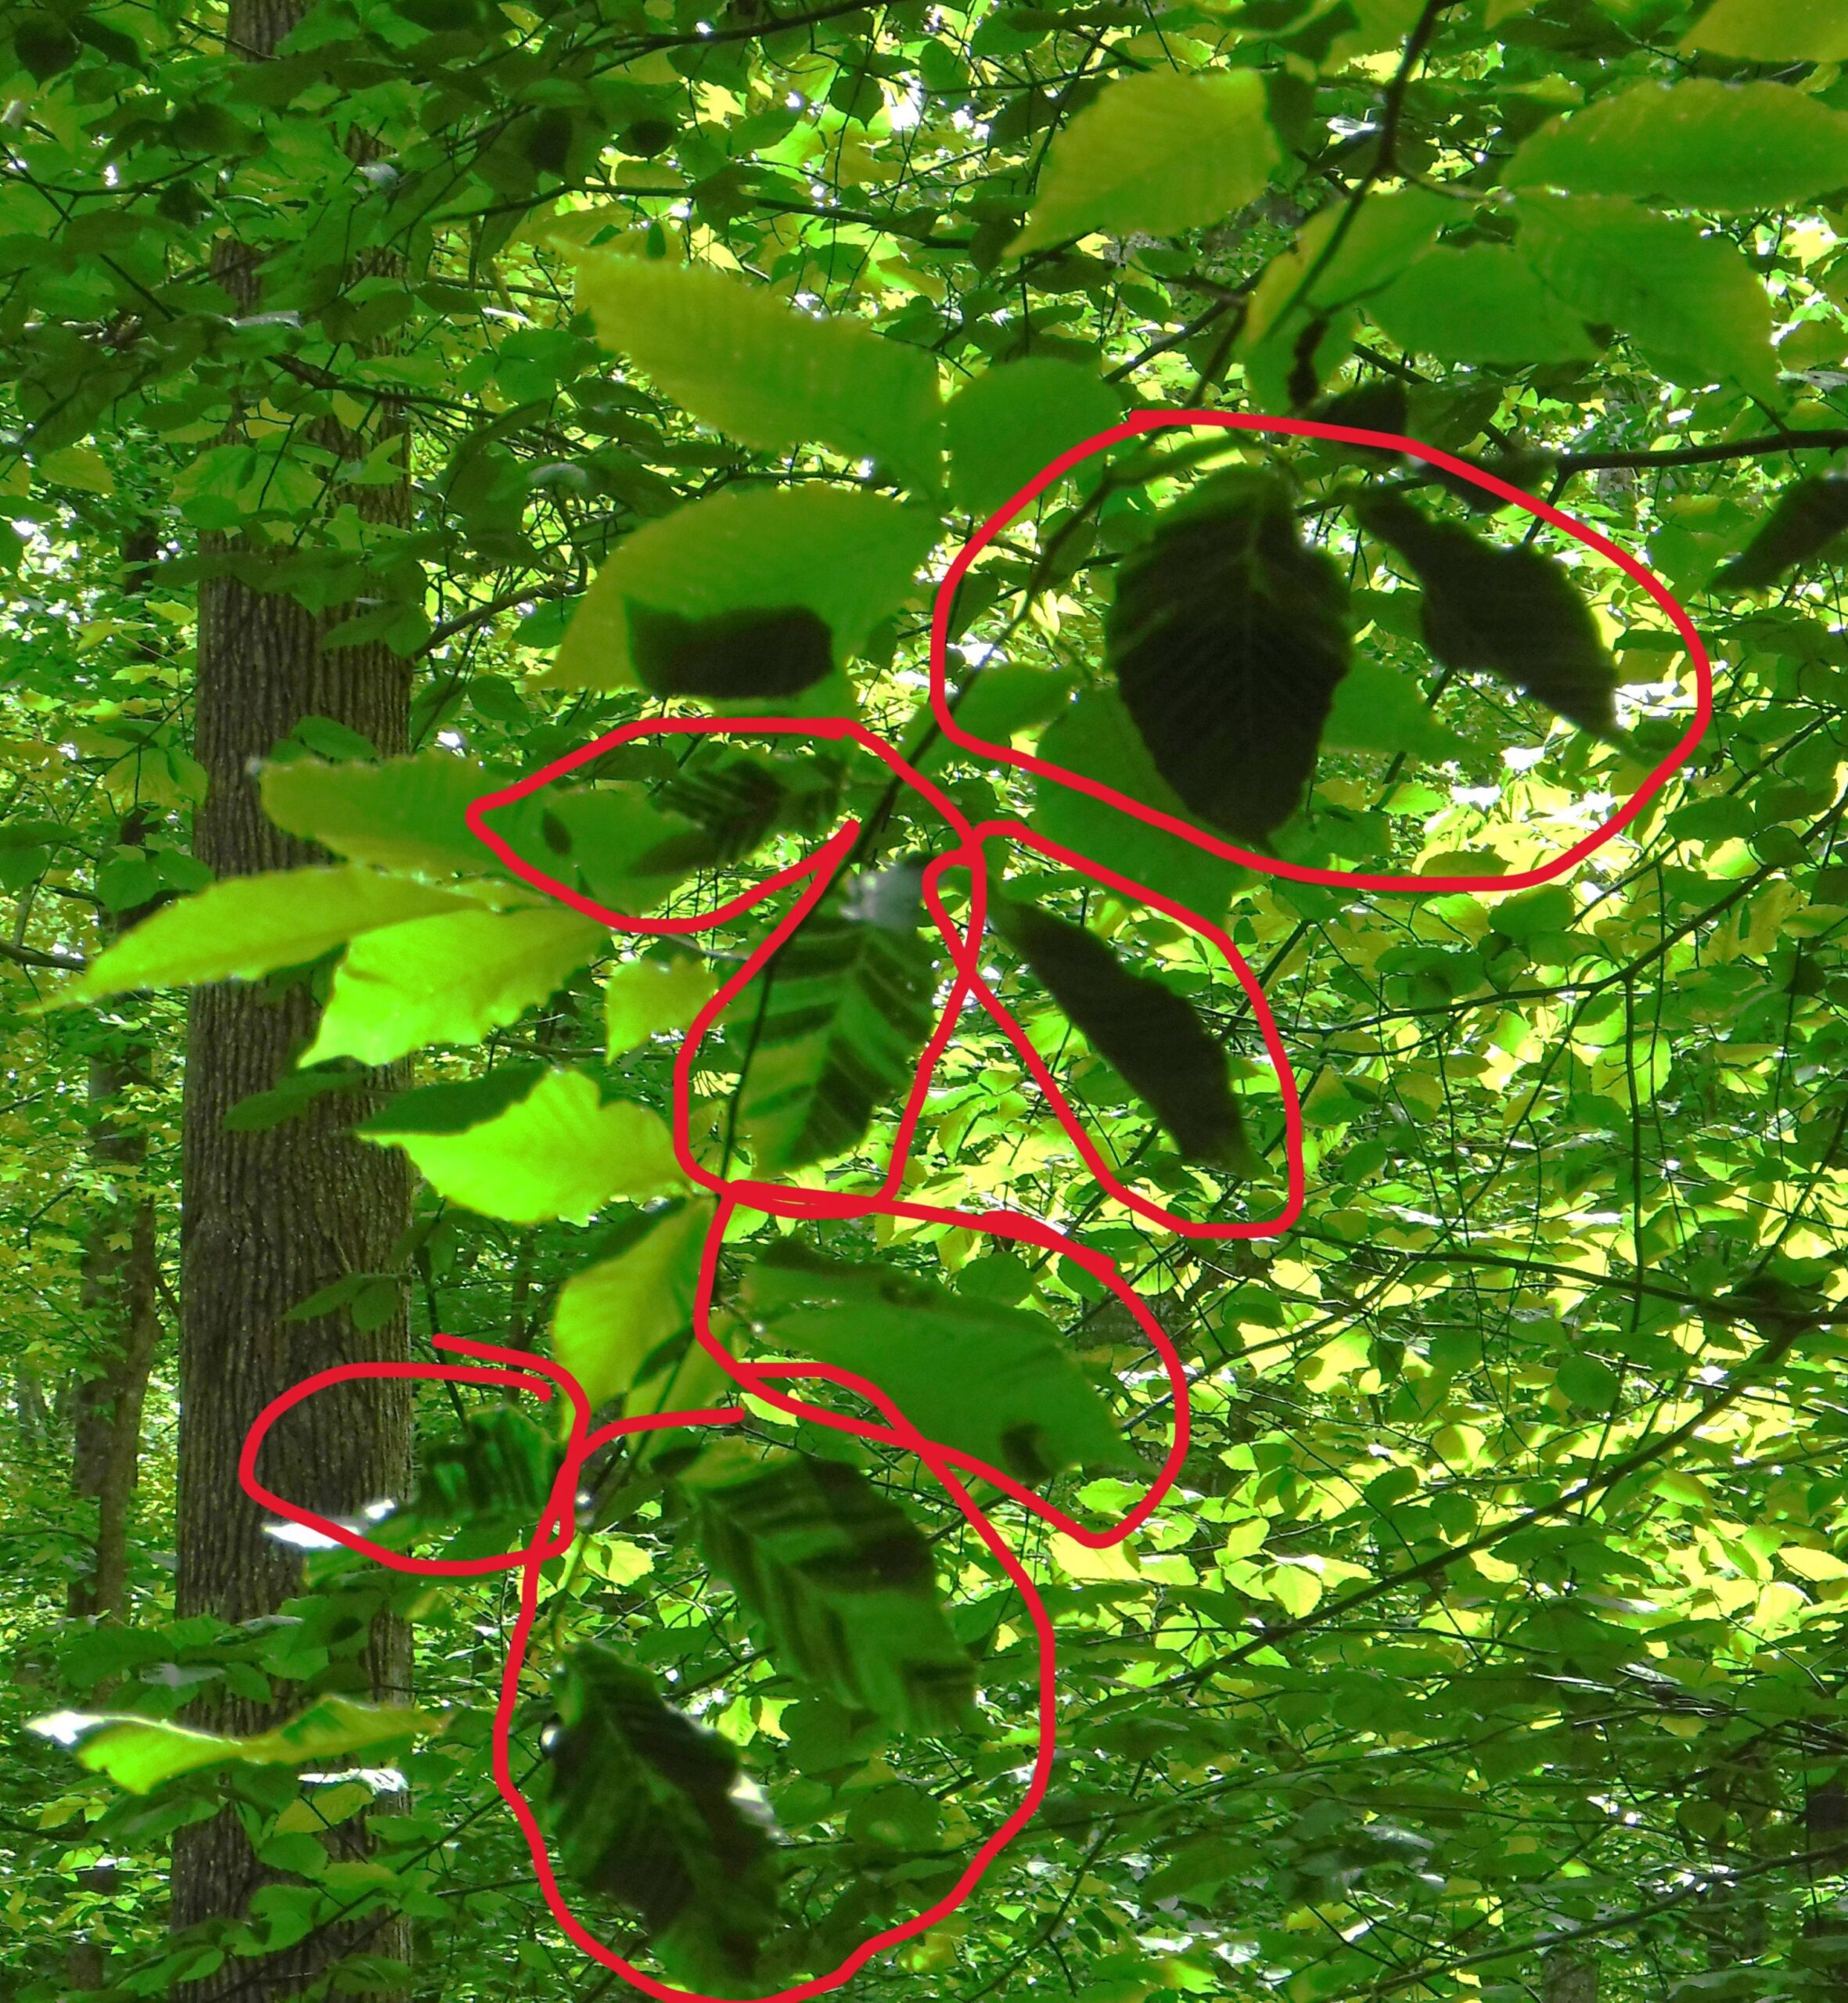
beech leaf disease symptoms, Fairfax County Virginia; photo by F.T.
To this list, I add beech leaf disease nematode (Litylenchus crenatae mccannii), the Euwallaceae/Fusarium complex, and, in Europe, lawson cypress root disease, along with numerous arthropods. These include emerald ash borer (Agrilus plannipennis), goldspotted oak borer (Agrilus auroguttatus), Erythrinagall wasp (Quadrastichus erythrinae). All have irreversibly shaped forest ecosystems in their introduced ranges. The forest losses have had numerous repercussions to human societies in the receiving regions.
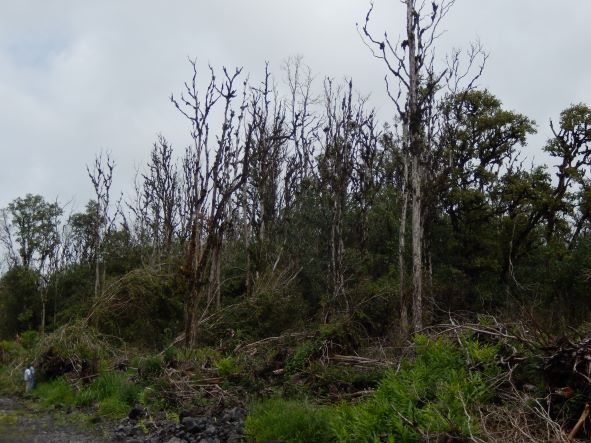
ohia trees killed by rapid ohia death; photo by Richard Sniezko, USFS
Mitigation Can’t Keep Up Due to System Failures
Tanney et al. 2025 opine that the inevitable conclusion is that past and current mitigation efforts have been insufficient to keep pace. Nor do the failures result only from growing volumes of imports that overwhelm inspection services.
They point to another reason: limited acknowledgment and integration of phytobiome-associated risks into regulatory frameworks. The system ignores particularly fungal endophytes and latent pathogens with extended asymptomatic or presymptomatic phases.
Their telling illustration is the ash decline epidemic in Europe. Hymenoscyphus fraxineus is a harmless endophyte–saprotroph on its native Asian host (Fraxinus mandshurica). However, it was introduced to the naïve host European ash (Fraxinus excelsior), on which it became an aggressive necrotrophic pathogen that has killed millions of trees. Even if the organism had been detected (the authors thought this unlikely) before the outbreak was recognized, the detection would not have triggered a risk assessment or any phytosanitary measures. None of the approximately 200 species in the genus had been reported as a pathogen. In fact, a congener, H. albidus, has a similar endophyte– saprotroph life cycle on European ash without causing harm.
McTaggart et al. (2016) flagged these issues a decade ago. They said that recent advances in gene sequencing technologies reveal a vast diversity of fungi causing asymptomatic infections. Some are endophytes, defined as fungi that, for all or part of their life history, asymptomatically colonize plant tissue. Some are pathogens with extended asymptomatic stages. When introduced to naïve hosts, some of either can erupt. Therefore, international phytosanitary measures, including the one significant effort to address the plants for planting pathway, ISPM#36, should focus more on phytobiomes as a biosecurity concern. (See my blog reporting Dr. Eliana Torres Bedoya on this topic.)
Tanney et al. (2025) are not alone in calling out the system’s failure. See Weed, Ayres, and Hicke (2013), Fei et al. (2019), Quirion et al. (2021) for North America; and Gougherty, Sitzia et al. (2021) and Martinac et al. (2025) for a global perspective. Raffa et al. (2023) say national and international phytosanitary policies and programs must reflect the true level of threat from introduced plant pathogens (of all Phyla and Kingdoms) and scientific limits.
Experts on ambrosia beetles – insects that have symbiotic relationships with fungi – say the same. Dell, Xu and Chi 2026 call for studies of Euwallaceae fornicatus’s broader phytobiome, especially bacterial communities, which are increasingly recognized as important components of the ambrosia beetle system.
Nor are Tanney et al. (2025) alone in calling on phytosanitary officials to stop using methods known to fail. That is, relying on visual inspections of plants and basing decisions on whether a pest has previously been designated.
A decade ago McTaggart et al. (2016) called for shifting from a name-based to a gene-based biosecurity risk mitigation approach. Burgess and Wingfield (2026) say officials must move beyond case-by-case responses to embrace broader preventative approaches that address the underlying mechanisms of pathogen emergence and spread.
As Tanney et al. (2025) and Bonello describe, the current international phytosanitary framework relies on symptomatic hosts carrying named pathogens. This approach ignores the facts:
endophytes and latent pathogens with prolonged asymptomatic phases are
ubiquitous – on and in leaves, buds, inflorescences, fruit, seeds, xylem, phloem, cambium, and bark. Phytobiomes are more species-rich on plants lacking disease symptoms.
diverse – fungi, bacteria, viruses, nematodes. Some are known pathogens.
challenging to identify. They often can’t be isolated using standard lab processes. If the genome has not already been sequenced and recorded in databases even sequencing-informative loci or barcodes might fail to identify the taxa. (Only ~150,000 species of an estimated 2.5 million fungi are so compiled.)
in some cases, a significant threat to forest health when introduced to naïve realms.
Scientists cannot predict impacts that might accompany introduction of nearly any of these organisms to a naïve host. Missing information pertains, inter alia, to endophyte identities and life histories, trees’ defenses, and the effects of the current and changing climate.
Host ranges might shift during an organism’s life cycle, e.g., juvenile vs. mature/reproducing.
Host jumps within the same host genus are likely (Tanney et al. 2025). They say that importing living plant into areas with congeneric endemic plants is highly risky.
Most endophytes in woody plants can be horizontally transmitted by abiotic (e.g., wind, rain, and surface water movement) transmission and biotic (e.g., insect) vectors. Every colonized leaf might be a propagule! (Tanney et al. 2025)
Microbes might reproduce both asexually and sexually. Sometimes dispersal of these propagule uses different modes, e.g., insect- and water-dispersed asexual spores combined vs. air-dispersed sexual spores.
Endophytes can switch from being asymptomatic to pathogenic when hosts are stressed. Tanney et al. (2025) name several examples, including Fusarium circinatum – causal agent of pine pitch canker.
To protect our plant resources – in forests, in agricultural fields, in our gardens – scientists must be empowered to develop methods and policies that better account for unnamed and unknown organisms.
Tanney et al. (2025) note that there is some flexibility in the face of unknown threats. The World Trade Organization’s Agreement on the Application of Sanitary and Phytosanitary Standards (SPS Agreement) and ISPM#2 allow adoption of a temporary phytosanitary measure based on the information available, even when it is limited. APHIS’ NAPPRA program link takes this approach. I think countries could use this flexibility more often. (I discuss the SPS and IPPC system in greater detail in my report Fading Forests II. I provide a link at the end of this blog.)
How to Improve Prevention
Some progress has been made in countering introductions of arthropods. Adoption of ISPM#15 regulates an entire pathway (crates, pallets, and other forms of packaging made from wood). CISP applauds the approach but calls for more aggressive enforcement. (On this website, scroll down below “Archives” to “Categories”, click on “wood packaging”). I note that introductions via this pathway nevertheless continue: Lantschner et al. (2026) have identified seven independent introductions of Euwallacea fornicatus. Introductions to San Jose, California; Israel; South Africa; Brazil; Spain; and Türkiye occurred after most countries had begun implementing ISPM#15. The same is true of the introduction of the congener E. kuroshio to southern California. Nardi et al. (2026) demonstrate continuing introductions of woodwasps in wood packaging.
Unlike wood products, imported plants, especially those intended to be planted in the new location, must remain alive and healthy. It is extremely challenging to devise effective treatments to kill the arthropod or pathogen without harming the plant. Tanney et al. (2025) discuss the pros and cons of several options, including ionizing radiation, fungicide treatments, and various heat treatments. They note that more research is needed to assess the feasibility, efficacy, optimal dosage, and potential risks of devitalizing plants in high-throughput treatments.
New Tools for Prevention
So the focus remains on preventing introductions. Fortunately, new tools make possible new approaches.
Detection of Pathogens — Tanney et al. (2025), Carnegie et al. (2026), Burgess and Wingfield 2026, and Bonello (pers. comm.) point to the suite of new molecular, remote sensing, and artificial intelligence tools becoming usable for detecting pathogens. They and Dell, Xu and Chi (2026) stress that citizen science can extend the reach of formal surveillance.
Rapid Responses — Tanney et al. (2025) and Carnegie et al. (2026) concede that more work is needed to address such considerations as detecting DNA from nonviable cells, and to develop international standards. However, they assert that results from these tools are already sufficiently science-based to inform decision-making, specifically to implement rapid responses including precautionary quarantines and other measures along with intensive surveys and conducting triage assessments.
Inspection and Enforcement — Burgess and Wingfield (2026) call more generally for enforcing comprehensive phytosanitary treatments and certifications for the live plant and timber trades, and focusing inspection efforts on high-risk entry points. Port detection can be sped up and improved by applying rapid molecular diagnostic tools.
Risk Assessments — New tools and approaches can also improve risk assessments. I blogged earlier about advances in predicting which trees are likely highly damaged, if certain pest insects are introduced. See Mech et al. 2019; Raffa et al. 2023; Schulz et al. 2025; Uden et al. 2022. This is encouraging, although additional work on arthropods is still needed. Carnegie et al. (2026) and Hulcr (2026, USDA Interagency Symposium on Invasive Species, Annapolis Maryland) both note the need for continued investment in taxonomic surveys to generate baseline data.
Predicting the probable impacts of introduced pathogens is inherently more difficult.
After introduction to novel systems pathogens sometimes evolve rapidly and becoming more aggressive and difficult to manage (Burgess and Wingfield 2026).
Host jumps within the host genus are likely. This exacerbates the risk arising from importing living plants into areas with congeneric endemic plants. Under these circumstances the risk assessment must be especially careful in balancing economic and social benefits of trade w/ potential ecological, economic, and social consequences of invasion (Tanney et al. 2025; Burgess and Wingfield 2026). Tanney et al. (2025) recommend systematic studies of regularly traded species from areas of origin (or sites of production) to eventual destinations to provide a foundation for assessing the risk of phytobiomes arriving on imported plants. These studies would also help to determine effectiveness of management approaches.
A number of authors are exploring how to address these difficulties. For example, Tanney et al. (2025) advise using “omics”-based approaches to predict invasiveness, virulence, and host interactions. Caveat: same genes are present regardless of whether the organism is an endophyte on its native host or a pathogen on a naïve host. At the same time, host response must be assessed by combining omics-based approaches, sentinel plantings, and modeling.
Tanney et al. (2025) also recommend greatly expanding sentinel planting-based surveillance. Sentinel plant systems must be carefully managed to provide the necessary levels of information. Raffaet al. (2023) nivemdiscuss strengths and weaknesses of this approach. Eliana Torres Bedoya and Enrico Bonello blog warn that sentinel plantings must support screening all plant parts, above and below-ground, for all potentially pathogenic taxa, including nematodes, phytoplasmas, and viruses. Furthermore, samples must be analyzed from asymptomatic plants, not just those showing signs of disease. Finally, samples must be collected throughout the year. Carnegie et al. (2026) call for greater coordination within the country and with international colleagues (e.g., through the International Plant Sentinel Network (IPSN).
Tanney et al. (2025) provide a convenient list of approaches they think will help close the knowledge gaps that challenge integrating attention to phytobiomes into phytosanitary decision-making.
Tanney et al. (2025) and Burgess and Wingfield (2026) advocate shifting the focus of risk assessments from specific pests to commodity-based or pathway risk assessments that consider unknown but plausible threats.
Horizon scanning is often described as helpful in predicting the next invasion. However, I have been disappointed by the usefulness demonstrated by some applications of the approach – at least in the absence of policies and resources to support a robust “rapid response”. At least in Cyprus blog and the United Kingdom, the main response to detection of one of the predicted species is only heightened monitoring — not attempted management!! According to Peyton et al. (2026), the British exercise failed to evaluate 78% of the 112 species that were introduced over the following decade. The vast majority were not evaluated because they were expected to have negligible impacts on biodiversity in Britain — but some turned out to be damaging.
Countries also need current data on which to base analyses and determine efficacy of programs. I regret that all American analyses of the risk associated with imported “plants for planting” rely on data collected by Liebhold et al. (2012) — which is from 2009!! Not only are these data 17 years old; APHIS has made major changes to its regulations in the interval — including implementation of the NAPPRA program.
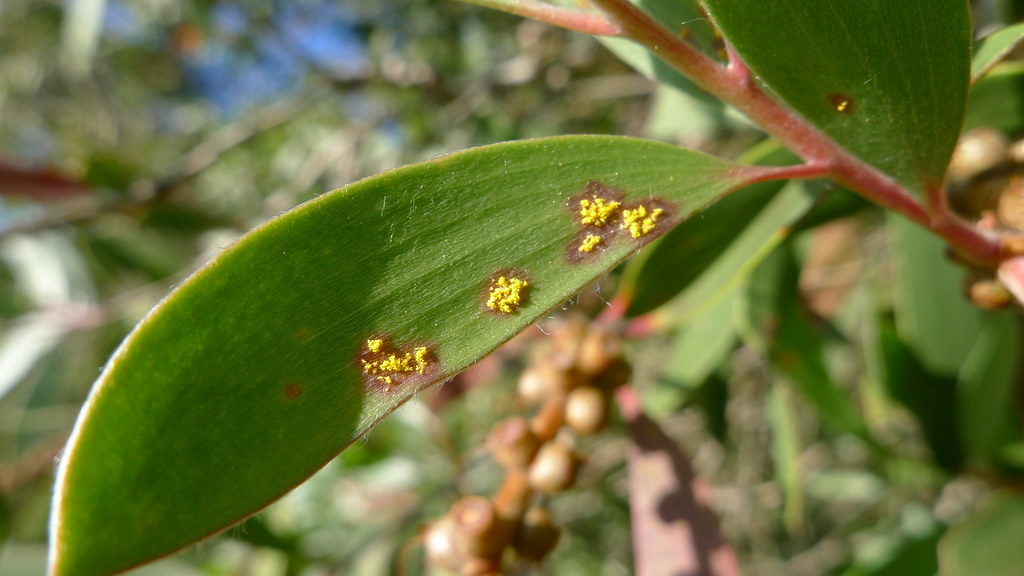
The missing component often is rapid response – often justified by uncertainty regarding the introduced organism’s possible impacts.Wingfield and Burgess (2026) cite the example of Australia’s weak response to detection of myrtle rust, Austropuccinia psidii. Now established in the rainforests of eastern Australia (states of New South Wales, Queensland, and Victoria) and an outbreak in Western Australia, myrtle rust threatens at least 76 species. Australia is home to 38% of all species in the vulnerable Myrtaceae family (Carnegie et al. 2026).
myrtle rust on Melaleuca tree in Australia; photo by John Tann via Flickr
Burgess and Wingfield (2026) cite several lessons based on the Northern Hemisphere’s experience with pathogen introductions. They call specifically for more stringent phytosanitary standards, advanced diagnostic techniques, and risk-optimized surveillance. These should be backed up by collaborative resistance breeding programs for high-risk hosts. They note the need for international cooperation across science, policy, industry, and communities.
Proposed Amendments to Trade Regulations
Tanney et al. (2025) point to the value of shifting to a system that favors trading in propagative material with subsequent bulking up in the importing countries for domestic consumption. (See also my advocacy in Fading Forests II.) They concede that this approach is unlikely to be implemented. As a fallback, they suggest applying this approach to the highest-risk commodities, e.g., rhododendron plants. They note that these plants have transported Phytophthora ramorum.
Scientific Fields
Burgess and Wingfield (2026) point to the need for multidisciplinary research to integrate forest pathology with chemical, ecological and social sciences to anticipate pest emergence. I add: integrating plant pathology with invasion science. The two disciplines rarely interact. Paap et al. (2020) suggest a framework to bridge this gap. I noted that the recent IUCN survey regarding the need for an updated species conservation strategy, while it incorporates invasive species issues, did not mention regional phytosanitary organizations, such as EPPO or NAPPO, among the bodies with whom invasions scientists should build relationships.
Interestingly, a group of experts on invasive plants (Hulme et al. 2026) are trying to expand relationships among researchers even more broadly. They seek to integrate invasion science into on-going discussion of global megatrends. Megatrends are clusters of interdependent global trends observed today that together have the potential to cause significant shifts in environmental, economic, and social conditions. At present, government, industrial, and other leaders evaluating how societies might adapt to these changes are not even considering their probable effect on bioinvasions. At least bioinvasion scientists are starting to evaluate the effects of the megatrends.
The invasion scientists explored how 15 megatrends might affect arrival, establishment, spread, and impacts (environmental and economic) of invading non-native plants over the next 25 years. They grouped the trends into four larger gigatrends: “Anthropocene”, “Digital”, “Societal”, and “Technology”.
They expect most of the megatrends to increase invasion risks, especially by accelerating species arrival and spread. While trends grouped under “Technology” promise some improvements in detection and control tools, there are significant barriers to their adoption. This worrying statement should be addressed by the proponents of applying these measures I cited earlier.
Hulme et al. (2026) urge invasion scientists to persuade policymakers that by taking decisive action to steer these trajectories toward mitigating the growing global threat of bioinvasion.
The Need for Adequate Funding and Political Support
Burgess and Wingfield (2026) note that risk assessment, inspection, detection, and response programs need to be supported by investment in quarantine infrastructure, diagnostic laboratories, and emergency response funds to enhance readiness for new incursions.
As they stress, prevention and preparedness cannot rest solely with scientists. Political commitment, regulatory authority, and industry engagement are indispensable. The efforts need the active participation of affected economic sectors, and sustained investment by governments, scientific institutions, industry, and society. The need for reliable, long-term funding and societal support is shared with all invasive species programs. Nearly all participants in the IUCN survey ranked this need at the top.
Property owners, the wood products and nursery industries, and governments from municipal to national have incurred substantial economic costs. Entire wooded ecosystems have been destroyed. Affected stakeholders, however, have not demanded that officials adopt more effective plant health strategies to reduce this risk. Scott Schlarbaum and I have released three “Fading Forest” reports trying to make this happen (links provided below). As shown here, many scientists are calling for action. To quote the late Congressman John Lewis in the context of civil rights, “If not now, when? If not you, who?”
SOURCES
Burgess, T.I. and M.J. Wingfield. 2026. Unveiling a Hidden Menace: Invasive Tree Pathogens, Less Known but Increasingly Threatening Southern Hemisphere Forests Annual Review of Phytopathology 64:18.1–18.2664:18.1–18.26
Carnegie, A.J., B.A. Summerell, C. Trollip F. Tovar, D.I. Smith, and J. McDonald. 2026. Sentinel trees for early detection of non-native forest pests and pathogens in Australia. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183
Dell, B., W. Xu, and N.M. Chi. 2026. Polyphagous Shot Hole Borer, a Global Threat to Forest Plantations, Green Infrastructure, and Biodiversity: Status, Challenges, and Solutions. Forests, 17, 832
Fei, S., R.S. Morin, C.M. Oswalt, & A.M. 2019. Biomass losses resulting from insect & disease invasions in United States forests
Gougherty, A.V. & Davis,T.J. (2024) Evolutionary history of host trees amplifies the dilution effect of biodiversity on forest pests. PLoSBio. 22(2):e30024730 https://doi.org/10.1371/journal.pbio.3002475 PLOSBiology |https://doi.org/10.1371/journal.pbio.3002473 February 27, 2024 1 / 1
Hulme, P.E., J.N. Barney, J.L. Bufford, J.A. Catford, J.A. Coetzee, C.C. Daehler, M.S. Dechoum, H. Jäger, A. Pauchard, P. Pyšek, D.M. Richardson, M. Vilà, E. Wandrag, J.R.U. Wilson. 2026. Seeds of change: Global megatrends will shape the future trajectory of plant invasions. BioScience , 2026, https://doi.org/10.1093/biosci/biag096
Lantschner, M.V., E. Ceriani-Nakamurakare, A.J. Johnson, A.I. Cognato, S.M. Smith, D.F. Gomez. 2026. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis (Coleoptera: Scolytinae), two global emerging pests. J Pest Sci 99, 100 2026. https://doi.org/10.1007/s10340-026-02070-w
Liebhold, A.M., E.G. Brockerhoff, L.J. Garrett, J.L. Parke, and K.O. Britton. 2012. Live Plant Imports: the Major Pathway for Forest Insect and Pathogen Invasions of the US. www.frontiersinecology.org
Martinac, M-L., F. Ningre, A. Dowkiw, N.Le Goff, B. Marcais. 2025. High host density favour ash dieback. Plant Pathology 2025, 74 (5) 10.1111/ppa.14099
Martinou, A.F., J. Demetirou, I. Angelidou, N. Kassinis, A. Melifronidou, J.M. Peyton, H.E. Roy, A.N.G. Kirschel. 2026. Multiple introductions of invasive alien species on a Mediterranean island predicted by horizon scanning. Biological Invasions 2026 28:41 https://doi.org/10.1007/s10530-025-03729-8
McTaggart, A.R., M.A. van der Nest, E.T. Steenkamp, J. Roux, B. Slippers, L.S. Shuey, et al. (2016) Fungal Genomics Challenges the Dogma of Name-Based Biosecurity. PLoS Pathog 12(5): e1005475. doi:10.1371/journal.ppat.1005475
Mech, A.M., K.A. Thomas, T.D. Marsico, D.A. Herms, C.R. Allen, M.P. Ayres, K.J. K. Gandhi, J. Gurevitch, N.P. Havill, R.A. Hufbauer, A.M. Liebhold, K.F. Raffa, A.N. Schulz, D.R. Uden, & P.C. Tobin. 2019. Evolutionary history predicts high-impact invasions by herbivorous insects. Ecology & Evolution 9(21): 12216–12230. https://doi.org/10.1002/ece3.5709
Nardi, D., K.E. Wagner, S.F. Ward, A.M. Liebhold, E.G. Brockerhoff, R.M. Turner, J.J. Riggins. 2026. Global movement of woodwasps (Hymenoptera: Siricidae) inferred from border interception records Biol Invasions (2026) 28:167 https://doi.org/10.1007/s10530-026-03881-9
Paap, T., M.J. Wingfield, T.I. Burgess, J.R.U. Wilson, D.M. Richardson, and A. Santini. 202 Harmonising the fields of invasion science and forest pathology NeoBiota Vol 62 2020 pages 301-332
Peyton, J.M., S. Rorke, D.C. Aldridge, O.L. Pescott, K. Dehnen- Schmutz, D.G. Noble, J. Sewell, A.J.A. Stewart, T. Adriaens, B.C. Beckmann, J. R. Britton, J. Brodie1, P.M.J. Brown, I.C.N. Cavadino, P.F. Clark, A.M. Dunn, J.Foster, C. Harrower, M.C. Harvey, M.C. Jackson, T. Jones, C.A. Maggs, G. Martin, F. Mathews, A.C. Mill, D. Murphy, E. Paganini, R. Payne, W. Rabitsch, T. Renals, K. Schönrogge, R.H. Shaw, G.C. Smith, P.D. Stebbing, P.A. Stroh, H. Tidbury, E. Tricarico, J. Vallet, K.J. Walker, L.E. Wood, C.A. Wood, B. Woodcock, H.E. Roy. 2026. Assessing the success of a horizon scanning approach in predicting invasive non-native species arrival. J Appl Ecol. 2026; 63: https://doi.org/10.1111/1365-2664.70217
Quirion BR, Domke GM, Walters BF, Lovett GM, Fargione JE, Greenwood L, Serbesoff-King K, Randall JM & Fei S (2021) P&P Disturbances Correlate With Reduced Carbon Sequestration in Forests of the Contiguous US. Front. For. Glob. Change 4:716582. [Volume 4 | Article 716582] doi: 10.3389/ffgc.2021.716582
Rabaglia, R.J., S.A. Dole, and A.I. Cognato. 2006. Review of American Xyleborina (Coleoptera: Curculionidae: Scolytinae) Occurring North of Mexico, with an Illustrated Key. Ann. Entomol. Soc. Am. 99: 1034–1056.
Raffa, K.F., E.G. Brockerhoff, J-C. Gregoirem, R.C. Hamelin, A.M. Liebhold, A. Santini, R.C. Venette, and M.J. Wingfield. 2023. Approaches to Forecasting Damage by Invasive Forest Insects and Pathogens: A Cross-Assessment. Bioscience Vol. 73, No. 2. February 2023.
Schulz, A.N., N.P. Havill, T.D. Marsico, M.P. Ayres, K.J.K. Gandhi, D.A. Herms, A.M. Hoover, R.A. Hufbauer, A.M. Liebhold, K.F. Raffa, K.A. Thomas, P.C. Tobin, D.R. Uden, A.M. Mech. 2025. What Is a Specialist? Quantifying Host Breadth Enables Impact Prediction for Invasive Herbivores Ecology Letters 28: e70083. https://doi.org/10.1111/ele.70083
Tanney, J.B., M. Kemler, M. Vivas, M.J. Wingfield, and B. Slippers. 2025. Silent invaders: the hidden threat of asymptomatic phytobiomes to forest security. New Phytologist 2025 247: 533–545 doi: 10.1111/nph.70209
Uden, D.R., A.M. Mech, N.P. Havill, A.N. Schulz, M.P. Ayres, D.A. Herms, A.M. Hoover, K.J.K. Gandhi, R.A. Hufbauer, A.M. Liebhold, T.D. Marsico, K.F. Raffa, K.A. Thomas, P.C. Tobin, C.R. Allen. 2022. Phylogenetic risk assessment is robust for forecasting the impact of European insects on No Am conifers. Ecological Applications 33(2): e2761. https://doi.org/10.1002/eap.2761
Weed, A.S., M.P. Ayers, J.A. Hicke. 2013. Consequences of climate change for biotic disturbances in North American forests. Ecological Monographs, 83(4), 2013, pp. 441–470
Posted by Faith Campbell
We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.
For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm
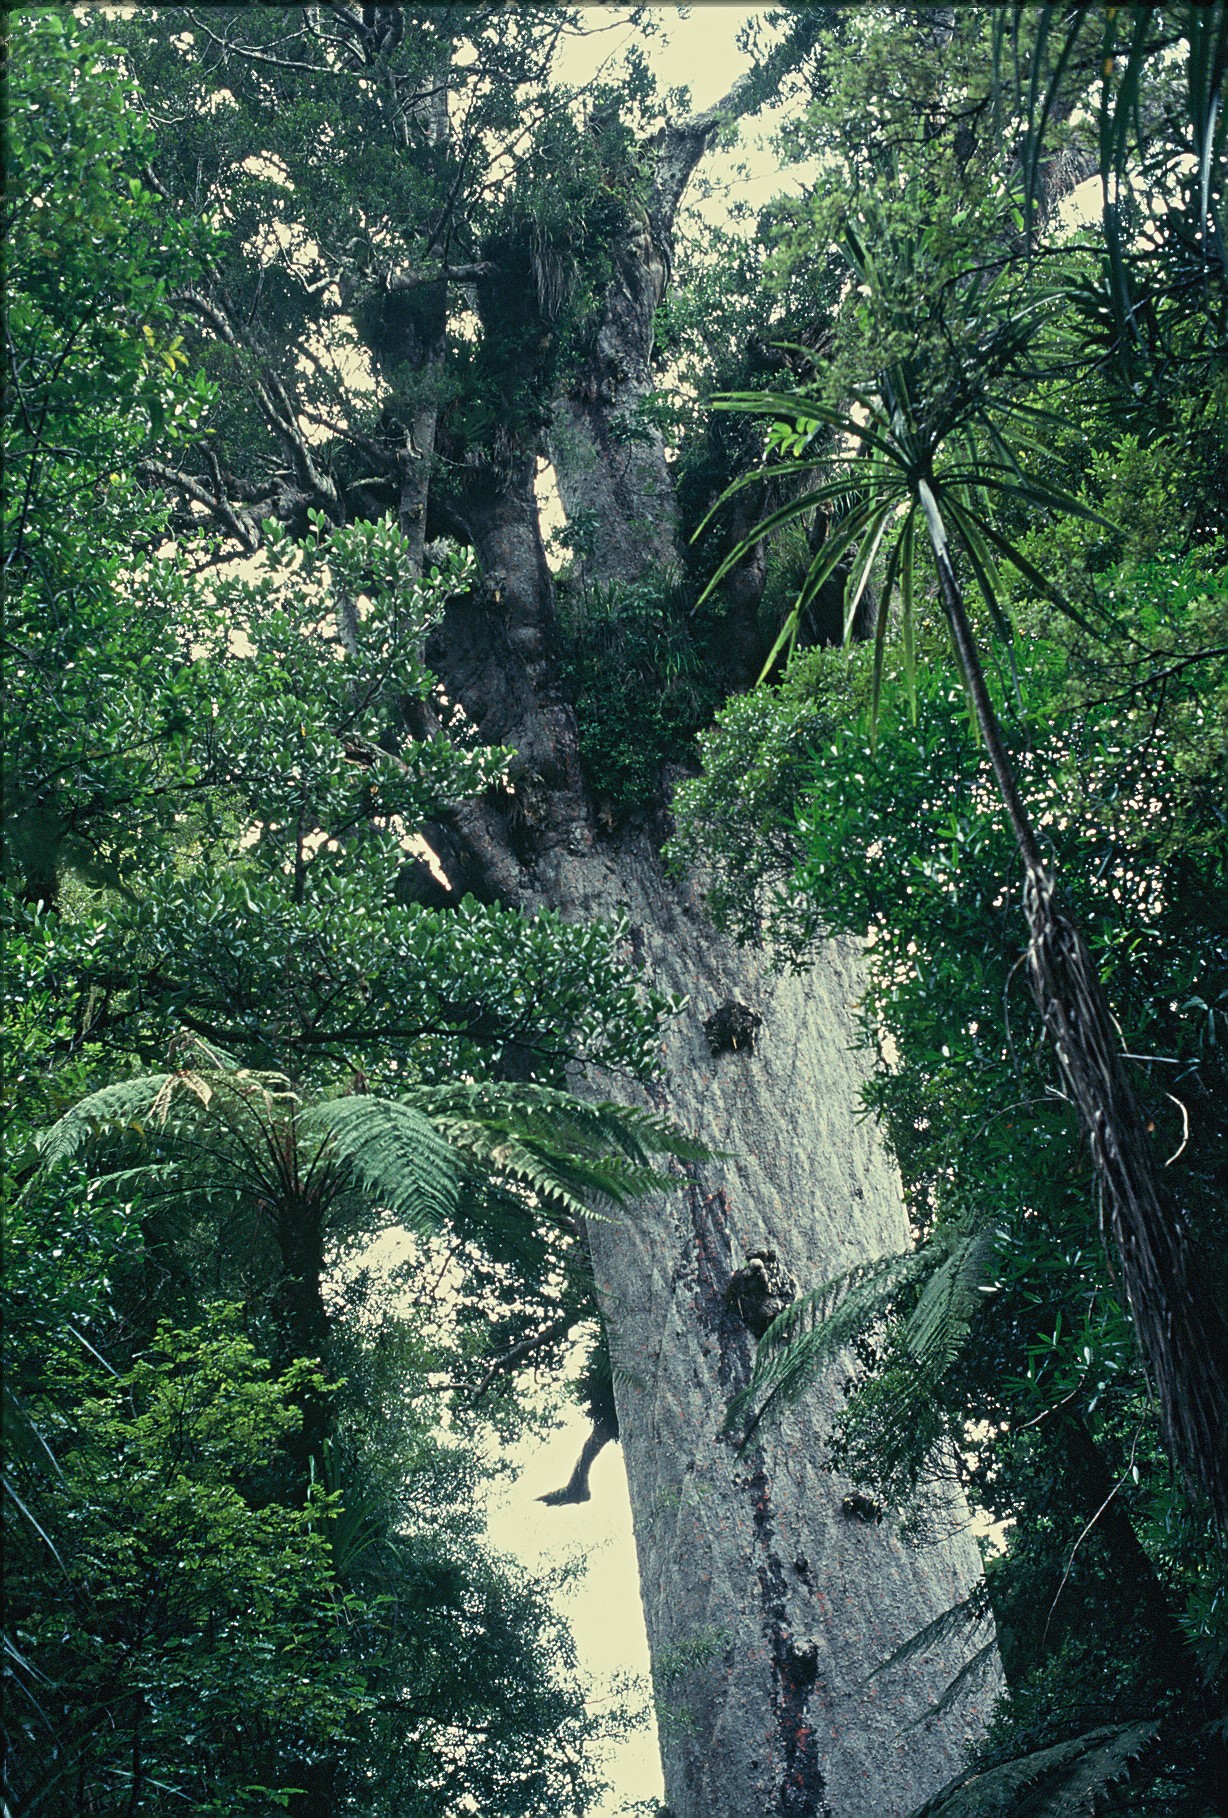
a large kauri tree on New Zealand’s North Island; photo by F.T. Campbell
I applaud the growing attention to the impacts of deadly pathogens in forests. The focus is often on the resulting decrease in tree-based storage of atmospheric CO2. In an earlier blog I cited findings by Quirion et al. (2021) that forest diseases in the United States between 2001 and 2019 reduced mean forest carbon sequestration by 28%. Forests were converted from carbon storage to carbon sources. [Full citations for all sources provided at the end of this blog.] Earlier, Fei et al. (2019) had determined that compensatory growth by non-host species (spurred by reduced competition and greater resource availability after a dominant tree species dies) might partially offset CO2 decline, although only over long timescales. Chan et al. (2026) cite examples from redwoods in California to Dipterocarps in Southest Asia that document the importance of large trees in sequestering atmospheric CO2. See also Calders et al. re: Wytham Woods in the United Kingdom.
A pertinent current example is found in New Zealand. There, the oomycete Phytophthora agathidicida is killing the endemic kauri tree, Agathis australis. Kauri are among the largest and longest-lived trees on Earth. The average age of large individuals in old-growth stands is ~ 600 years; exceptional specimens reach 1,600 years. Typical diameters in old-growth stands are 1.3–1.5 m; exceptional specimens > 7 meters (Chan et al. 2026).
A year ago Simpkins et al. (2025) reported a modeling study that indicated that kauri dieback disease could cause a decrease in aboveground carbon stocks by 55% over 500 years. However, as Chan et al. (2026) point out, stand-level carbon sequestration and storage in a forest undergoing widespread mortality of the dominant tree species depend on growth and productivity of the replacement species. Even the magnitude of short-term dynamics depends on the relative abundance of the vulnerable host and the rate of its mortality and decline.
Therefore they explored the impact of kauri dieback in greater detail, including which species they thought likely to replace kauri and their carbon-sequestration capabilities at the stand level.
Although (regrettably) not the focus of their article, Chan et al. (2026) note that loss of the kauri tree also threatens biodiversity. Kauri strongly modify their environment through accumulation of a thick organic soil layer derived from litter. The layer is typically 30 to 50 centimeters deep but can reach 2 meters. These soils are acidic, drought-prone and nutrient-poor. As result the co-occurring plants comprise a unique suite of stress-tolerant plants. The vertical stratification of conifer and angiosperm crowns in kauri forests allows coexistence and unusually high total basal area of other plant species.
In these forests, kauri have dominated annual CO2 capture and long-term storage. Under pre-invasion conditions, Chan et al. (2026) this to continue. Previous work estimated that live vegetation biomass in kauri stands doubles when the stand moves from early- or mid-successional stages to mature. Three other species each contribute more than 10% of carbon storage: the tree fern Cyathea dealbata, and two small trees, Phyllocladus trichomanoides and Kunzea ericoides. All are early successional species that typically dominate in open or disturbed environments but decline as canopies close.
Chan et al. (2026) studied changes in live vegetation carbon stocks between two census periods ten years apart, 2011 – 2014 and 2021 – 2024. The five kauri-dominated plots included two plots each in early- and late-successional stages and one mid-successional stand. The study site was in the greater Auckland region of North Island. Phytophthora agathidicida is spreading through these forests, infecting kauri of all ages. Still, dieback intensity varies within the plots, so they were subdivided plots into 20 10 m × 10 m subplots.
Chan et al. (2026) tried to measure two distinct processes: the increase in carbon stocks coming from recruitment and growth of live stems (= productivity) and loss of sequestration and storage due to tree mortality. The two phenomena might respond differently to kauri dieback and initial carbon stocks. While increasing disease severity and increased mortality both result in lower net accumulation, it is important to disentangle the effects of increased loss, reduced productivity, or the combination.
kauri killed by dieback disease; 149 kauri dieback 02-868×1300
Findings
Carbon sequestration declined proportionately with increasing disease severity due to both reduced productivity and greater carbon loss from mortality. Because kauri contributed the largest share of carbon sequestration and storage due to the enormous size of some individuals, death of higher numbers of large kauri led to the largest reductions in these services. That is, the greatest observed decrease in carbon sequestration and storage was in those stands that initially had the highest levels of carbon storage. These were stands in mid- and late-successional subplots rather than in early-successional subplots. The higher the initial mean carbon stock level, the more pronounced the observed decline in sequestration.
This means that kauri dieback threatens both the carbon sequestration and long-term carbon storage capacity of kauri forests, particularly in mature stands comprising the largest trees.
Chan et al. (2026) conclude that the carbon stocks of these mature kauri stands will not stabilize until after substantial depletion of kauri biomass. As a result, long-term carbon storage capacity is markedly reduced.
Meanwhile, healthy kauri stands continued to sequester carbon as the trees grew. Chan et al. (2026) expect living kauri trees to continue adding to their basal area and other productive species can co-exist under the vertically stratified crowns.
In stands that had low carbon sequestration levels at the time of the first census (early successional stands), the stand maintained positive carbon sequestration until the disease reached a higher intensity. This was because some of the other tree species in the stand raised their proportional contributions to CO2 sequestration. Chan et al. (2026) concluded that these stands were likely stabilize at a reduced level of biomass, effectively lowering their long-term carbon storage and sequestration potential.
The steep decline in carbon sequestration and storage associated with higher initial carbon stocks reveal the disproportionate vulnerability of mature kauri stands. The kauri contribution to stand biomass is unlikely to be replaced by a structurally similar species, e.g., the long-lived, large conifer rimu (Dacrydium cupressinum), until passage of many years. Early-successional species are expected to colonize the damaged forests rapidly, but their lower wood densities and fast maturity/senescence confer limited carbon storage capacity.
a rimu tree; photo by F.T. Campbell
Besides, some of the species likely to replace (temporarily) dead kauri — Myrtaceae such as Kunzea ericoides — are susceptible to another introduced pathogen, myrtle rust (Austropuccinia psidii) (Lantham et al. 2025).
So kauri dieback not only reduces current carbon stocks but succession dynamics do not support future sequestration potential, leading to a long-term decline in the carbon storage capacity of these forests.
Chan et al. (2026) call for urgent efforts to prevent spread of the pathogen Phytophthora agathidicida and injection of phosphite to reduce disease symptoms. Both strategies should target mature kauri stands. Research on phosphite treatments is under way. They also suggest research on disease progression and associated changes in carbon stocks across multiple pools, including coarse and fine woody debris and deep organic soil layers.
Chan et al. (2026) report that the disproportionate contribution of large, long-lived individual trees to carbon storage is a worldwide phenomenon.
Extraneous thought: I am glad that Chan et al. (2026) cite examples of high-impact pathogens from the Southern Hemisphere, i.e., Phytophthora cinnamomi in Australia. While chestnut blight certainly had severe impacts, so have many others, e.g., white pine blister rustCronartium ribicola. Some arthropods have also proved damaging on several continents, including emerald ash borer (Agrilus plannipennis), or across widely separated island systems, e.g., Erythrinagall wasp (Quadrastichus erythrinae) and cycad scale (Aulacaspis yasumatsui). I regret that I can find no recent information on the scale.
SOURCES
Calders, K., H. Verbeeck, A. Burt, N. Origo, J. Nightingale, Y. Malhi, P. Wilkes, P. Raumonen, R.G.H. Bunce, M. Disney. Laser scanning reveals potential underestimation of biomass carbon in temperate forest. Ecol Solut Evid. 2022;3:e12197. wileyonlinelibrary.com/journal/eso3
Chan, P.J., T. Elliott, H.R. Lai, B. Burns, L. Schwendenmann. 2026. Consequences of a dieback disease on carbon stocks and fluxes in forests dominated by a susceptible foundation species. Plant Ecology (2026) 227:97 https://doi.org/10.1007/s11258-026-1669-4
Fei, S, R.S. Morin, C.M. Oswalt, and A.M. Liebhold. 2019. Biomass losses resulting from insect and disease invasions in US forests. Proceedings of the National Academy of Sciences. August 27, 2019 vol. 116 no. 35 www.pnas.org/cgi/doi/10.1073/pnas.1820601116
Latham, M.C., A. Lustig, N.M. Williams, A. McDonald, T. Patuawa, J. Chetham, S. Johnson, A. Carrington, W. Wood, and D.P. Anderson. 2025. Design of risk-based surveillance to demonstrate absence of Phytophthora agathidicida in NZ kauri forests. Biol. Invasions (2025) 27, no.26 https://doi.org/10.1007/s10530-024-03501-4
Quirion BR, Domke GM, Walters BF, Lovett GM, Fargione JE, Greenwood L, Serbesoff-King K, Randall JM and Fei S (2021) P&P Disturbances Correlate With Reduced Carbon Sequestration in Forests of the Contiguous US. Front. For. Glob. Change 4:716582. [Volume 4 Article 716582 doi: 10.3389/ffgc.2021.716582
Simpkins, C.E., P.J. Bellingham, K. Reihana, J.M.R. Brock, G.L.W. Perry. 2024. Evaluating the effects of two newly emerging plant pathogens on North Aotearoa-NZ forests using an individual-based model. Ecological Modelling, www.elsevier.com/locate/ecolmodel https://doi.org/10.1016/j.ecolmodel.2024.110938
Posted by Faith Campbell
We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.
For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm
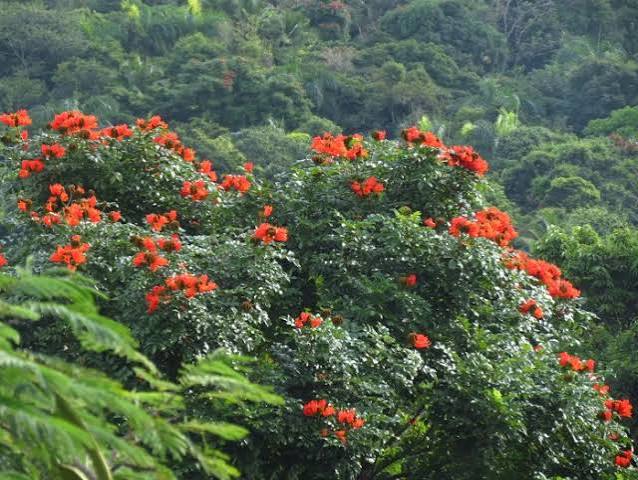
Spathodea campanulata (one of the most common invasive plant species in moist or wet forests on Puerto Rico); photo by Annika Lindqvist via EasyScape
America’s Caribbean islands have received much less attention that Hawai`i with regard to either their biological importance or level of biological invasion. I posted a blog three years ago about invasive tree species. I rejoice that the silence might be starting to change – thanks in large part to Julissa Rojas-Sandoval.
The West Indies
The Caribbean islands – including but not limited to Puerto Rico and the U.S. Virgin Islands – are considered one of 35 global BD hotspots on Earth (Castro, Quinones, and Gould 2016; Zimmerman et al. 2021). The most comprehensive descriptions are a decade old. Castro, Quinones, and Gould (2016) report that the Caribbean islands are home to ~14,526 plant and terrestrial vertebrate species, half of which are endemic to the region. At that time more than 900 species were on the IUCN Red List. The West Indies are characterized by exceptionally high levels of plant endemism, with more than 70% of seed plants considered endemic to the region (Rojas-Sandoval et al. 2017, citing earlier floristic assessments).
The Caribbean islands have a long history of anthropogenic disturbance – especially since Europeans arrived in 1492 — and intentional or accidental introductions of non-native species. Available sources differ on the number of species that should be categorized as “invasive”.
Potteret al. (2022) report that 17% of the flora of the islands of the Caribbean archipelago are not native. Rojas-Sandoval et al. (2017) identified 516 invasive non-indigenous plant species, representing about 4% of the total West Indian flora, and concluded that the incidence of invasive plants in the region is high compared with other island groups. Interestingly, each island group has its own suite of invasive species. More than 60% of these taxa occur on a single island. Thirty-eight percent belong to one of three families — Fabaceae, Poaceae, and Asteraceae. Thirty-four families are represented by a single species; 78 families by fewer than five.
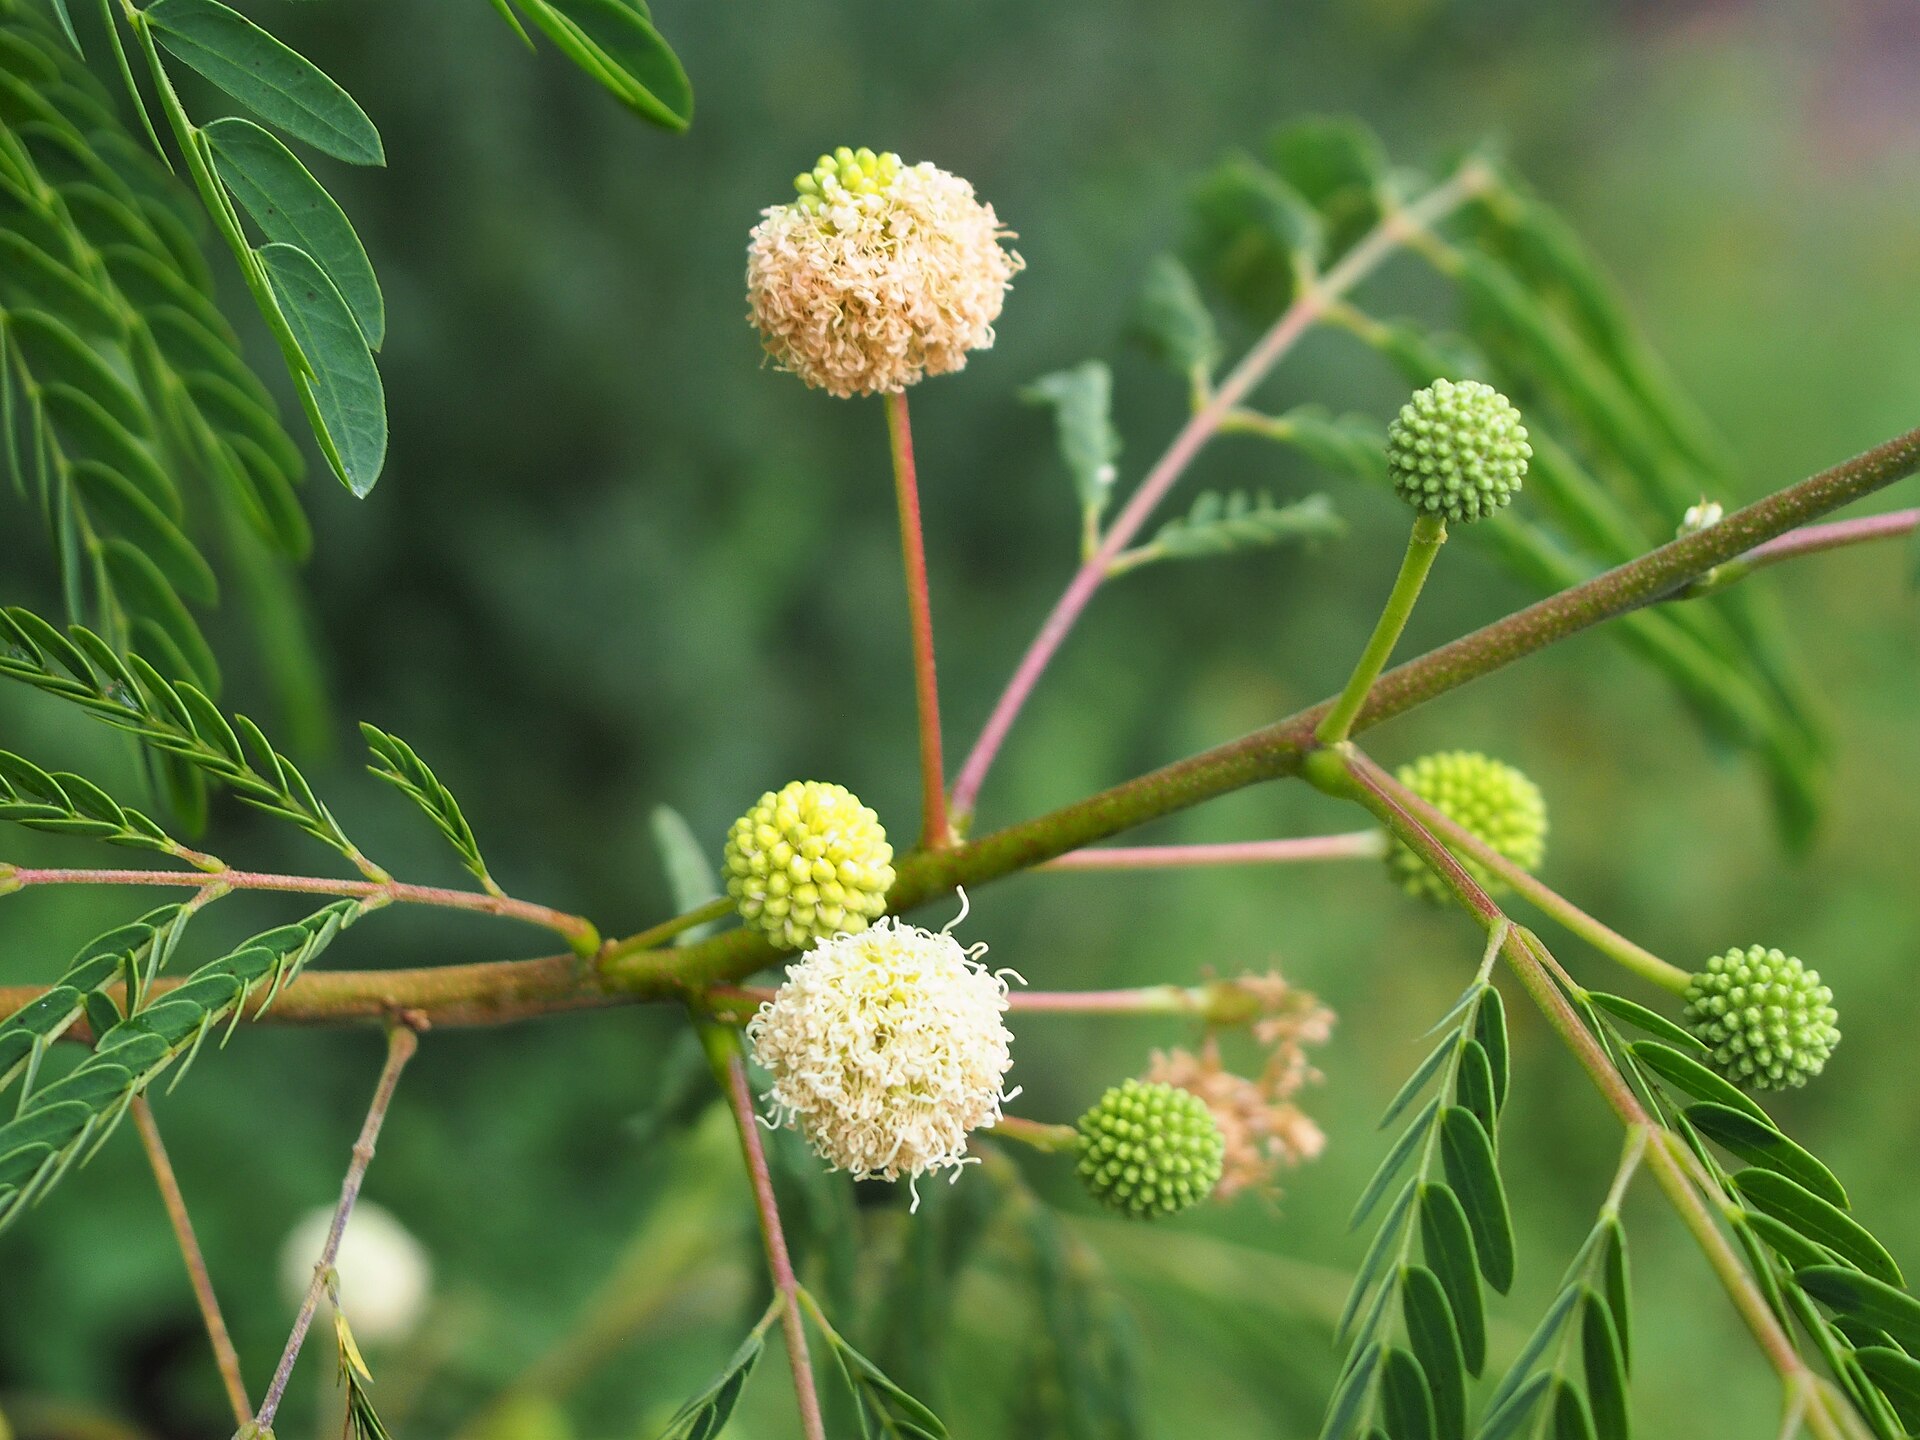
Leucaena lecocephala; photo by Agnieszka Kwiecien-Nova via WikiMedia
They report that the most widely distributed species is river tamarind, Leucaena leucocephala (Fabaceae); it occurs on all nine islands. Another seven species are found on seven of the islands: Casuarina equisetifolia (Casuarinaceae); Eichhornia crasssipes (Pontederiaceae); Megathyrsus maximus (Poaceae); Melaleuca quinquenervia (Myrtacea); Ricinus communis (Euphorbiaceae); Spathodea campanulata (Bignoniaceae), Terminalia catappa (Combretaceae).
The density of invasive plants per square kilometer varies considerably among the islands. The Virgin Islands (US and British) rank second highest at 0.245 / km2. Puerto Rico doesn’t stand out. As noted above, each island has a distinct invasive flora. The pair of islands which share the highest number of species (122) is Puerto Rico and the Virgin Islands (Rojas-Sandoval et al. 2017). I suggest it might be informative to explore whether these islands’ century-long ties to the United States influenced trade pathways and planting choices, thereby leading to this similarity.
Rojas-Sandoval et al. (2017) report that 31% of the invasive plants (162 species) are herbs; 20% (102 species) are trees; 16% (80 species) are shrubs; 15% (77 species) are grasses; 13% (67 species) are vines; 3% (15 species) are succulents; 2.5% (13 species) are aquatics. Three-quarters are perennials. These plants occur primarily in human-altered habitats: 98% (506 species) in ruderal areas; 61% (314 species) in seminatural areas; 35% (138 species) in agricultural areas. Only 5% (27 species) are found in mature forests.
Nineteen of the species are listed among the “world’s worst alien invasive species”. For example, six of the eight most widely distributed species (above) are invasive in Florida also.
Seventy-five percent of the invasive plant species have escaped from cultivation. According to Rojas-Sandoval et al. (2017), half of these were introduced as ornamentals; another third were introduced for various agriculture and forestry purposes. Finally, 7% were deliberately planted in natural ecosystems for some purpose such as erosion control. They suggest that repeated introduction of some of these species – especially the ornamentals – might increase propagule pressure and thus their probability of establishing.
Generalities About Biology on Puerto Rico
Puerto Rico is the smallest island of the Greater Antilles at ~ 9100 km2 (5,325 mi² / 1,379,000 ha) (Rojas-Sandoval, Presley, and Willig 2026). It is 39% forest, 32% grassland, 13% woodland and shrubland, 11% urban, 3% herbaceous wetlands, 1% forested wetlands, 1% inland water, < 1% natural barrens (Castro, Quinones, and Gould 2016).
Puerto Rico is relatively poor in species richness compared to mainland tropical areas. In one example, a plot in a Puerto Rican wet forest had half the number of freestanding woody species as a comparably-sized area in central Panama. Puerto Rico lacks large herbivores and predators. Still, Puerto Rico is much more diverse than other more isolated islands, e.g., the Hawaiian Islands (Zimmerman, Rojas-Sandoval, and Shiels 2021). There are 2,780 species of plants and 361 native vertebrates, including 277 birds, 52 reptiles, 19 amphibians, and 13 mammals (Castro, Quinones, and Gould 2016).
This biodiversity reflects the island’s highly varied topography – elevations range from sea level to 1338 m – and rainfall. Areas in the south and southwest receive ~800 mm while the high-elevation areas in the northeast are drenched by more than 4000 mm.
Unlike in most tropical areas, forests on Puerto Rico are regrowing due to abandonment of agriculture. Forest cover has increased from less than 6% in the 1950s to more than 55% by 2014. These regenerating forests contain a mixture of native and non-native species in a mosaic of forest at various stages of succession (Rojas-Sandoval, Presley, and Willig 2026). Potteret al. (2022) reported that two-thirds of Puerto Rico’s forests comprised novel tree assemblages.
Invasive species
A decade ago, Puerto Rico had 176 invasive plant species – 32% of the island’s flora. They comprised 44 herbs, 35 grasses, 33 trees, 28 vines, 19 shrubs, and 5 succulents. In this category, Puerto Rico ranks higher than other islands in the Greater Antilles e.g. Jamaica (21%), Dominican Republic (18%), and Cuba (12%) (Rojas-Sandoval et al. 2017; Rojas-Sandoval and Acevedo-Rodríguez 2015).
Three studies have addressed invasive species on “la Isla del Encanto”. They differ in in geographic scope, data, and study objectives.
Zimmerman, Rojas-Sandoval, and Shiels (2021) addressed biological invaders in all taxonomic groups, not just vascular plants. However, their analysis was limited geographically to the Caribbean National Forest (CNF; popularly known as El Yunque). This study was based on published literature, museum and herbarium collections, local and academic experts’ experience, and personal field observations. They concluded that there were some worrisome trends but no strong evidence that the National Forest’s ecosystem was in danger of fundamental change as a result of invasive species. However, they admit data were limited and called for systematic surveys and detailed studies. This need is particularly acute because of the ecological importance of El Yunque, which is one of the few (and the most important) remnants of original native forest on Puerto Rico.
Potter et al. (2022) relied on data collected as part of the USFS Forest Inventory and Analysis (FIA) survey. The survey evaluates 341 permanent plots every 5 years. They assessed trees (no other kinds of plants) in forested areas across the island, not just in the CNF. They usually attribute invasive trees’ prevalence largely to the land-use history, i.e., reforestation of formerly agricultural lands. These scientists emphasize the importance of recent land-use history in determining where non-native tree species occur. They do not offer an overall assessment of the trajectory of invasions.
A more recent analysis by Rojas-Sandoval, Presley, and Willig (2026) was also island-wide and included all woody plants with dbh ≥ 2.5 cm, i.e., trees and shrubs. Noting that invasion intensity is steadily increasing in Puerto Rico’s forests, they concluded that the threat to Puerto Rico’s native biological diversity is greater than did the earlier studies.
Relying on the FIA surveys has the advantage of providing statistically valid data. However, this survey has two drawbacks as regards assessing plant invasions. First, the FIA inventory data don’t evaluate species in the understory, i.e., herbs, small shrubs, or vines. These species might also alter long-term successional trajectories (Rojas-Sandoval, Presley, and Willig (2026). Second, the FIA inventory is not designed to detect even woody plant species in the early stage of invasion, i.e., those that occur only as small seedlings on a few inventory plots (Potter et al. 2022).
El Yunque
Invasive Plants
Zimmerman et al. (2021) report that 168 non-native plant species from 135 genera and 57 families are established in the National Forest – at varying levels from “naturalized” to fully invasive. Of these, 77 species (~46%) had previously been listed as invasive on Puerto Rico. Twelve were hangers-on from crops planted in the past (e.g., coffee, mango, and breadfruit). They considered most of these non-invasive because they hadn’t increased strongly during a 10-year study. They named one possible exception, Simarouba amara, a timber tree, which had increased in numbers in areas of less intense land use after hurricanes in late 1990s. However, this species has not been mentioned as problematic by any other study.
El Yunque (CNF) is home to 37 of the non-indigenous plant species, including 14 vines, nine herbs, and eight grasses. These plants are described as colonizing primarily disturbed areas (e.g., landslides), wastelands, river edges, and roadsides.
The non-native species present in the regrowing forests vary by forest type – as would be expected given the large differences in rainfall. In the subtropical dry forest the principal invasive plants are river tamarind (Leucaena leucocephala) and Prosopis juliflora (Rojas-Sandoval, Presley, and Willig (2026). The former is one of the most widespread and common of the highly invasive non-native tree species throughout the Caribbean. On Puerto Rico, L. leucocephala is documented on 12.6% of 294 forested plots, 40% of plots in this biome. P. pallida (algarroba) is recorded on 10.9% of all survey plots, 27.1% of plots in the biome. Invasions in the dry forest are sometimes arrested by chronic disturbance – presumably fire (Potter et al. 2022). However, the authors do not report which species – native or introduced – come in after the disturbance.
The subtropical moist forest is presumably the biome most affected by previous agricultural efforts. African tuliptree (Spathodea campanulata) occupies 41.8% of survey plots in this biome. Rose apple (Syzygium jambos) is found on 36.4% of these survey plots (Potter et al. 2022).
Invasive trees in the subtropical wet and rain forests biome included Erythrina poeppigiana and two species also found in the moist biome – Spathodea campanulate, and Syzygium jambos. S. campanulata is found on 33.9% of the plots in this biome (Potter et al. 2022). Zimmerman et al. (2021) call our attention to an herb, Selaginella willdenowii. They call this ornamental spikemoss one of most aggressive plant invaders in the CNF.
There is a difference of opinion on the threats posed by Spathodea campanulata. Potter et al. report that S. campanulata is found on 6.1% of all plots surveyed – half or less of plots invaded by the dryland species Leucaena leucocephala and Prosopis juliflora (and the S. campanulata plots are spread across two much larger biomes – moist and wet forests). S. campanulata is also shade intolerant so Potter et al. believe it might decline in the future as other species overtop it. The conflicting opinion is offered by Rojas-Sandoval, Presley, and Willig (2026). They call Spathodea campanulata a key driver of native biodiversity loss and homogenization in moist and wet forests. They note that the species has broad ecological tolerance and can proliferate after hurricanes. They found the species to already be significantly influencing native forest distinctiveness and composition – and to be increasing in abundance.
Potter et al. (2022) considered rose apple (Syzygium jambos) to pose a higher threat since it is shade tolerant and can form dense, monotypic stands under closed canopies – which S. campanulata cannot. Zimmerman, Rojas-Sandoval, and Shiels (2021) agree that where it occurs in areas of secondary forest near stream beds, S. jambos outcompetes other species. Rojas-Sandoval, Presley, and Willig (2026) note the species might potentially contribute to homogenizing biodiversity. A new development might counter this threat: the accidental introduction of guava/ohia rust (Austropuccinia psidii); it has been highly fatal to rose apple populations in Hawai`i. Both Zimmerman et al. and Rojas et al. mention this possibility but I have not seen a more recent discussion of whether this is occurring.
myrtle rust on Syzygium jambos; photo by Smallbiologie via Wikimedia
Zimmerman et al. (2021) say several invasive vines are established in El Yunque. The vines respond quickly to the disturbances caused by the region’s frequent hurricanes. Seven of the 14 species in the CNF are morning glories in the Ipomoea genus. Other locally abundant non-native vines are Epipremnum pinnatum, Pueraria phaseoloides, Dioscorea alata, Thunbergia alata, and Thunbergia fragrans.m
Potteret al. (2022) defined invasive tree species as those exhibiting 60 – 75% of stems in the “small” diameter categories (less than 12.5 cm dbh). Fifty-seven non-native tree species in old-growth and regenerating forests it this definition. They considered 17 of them as highly invasive, 16 as potentially highly invasive, and two as moderately invasive. That is, 35 of 57 nonnative tree species, or 60%, are actually or potentially bioinvaders. While on the continent only seven non-native tree species occurred on at least 2% of FIA plots across the ecoregions in which they were inventoried, on Puerto Rico 21 species (38%) occurred on at least 2% of the FIA plots. Potter et al. (2022) could not assess the invasiveness of eight additional species that occurred only as small stems on a couple of survey plots.
Potter et al. (2022) note the possibility of conflicting views about the invaders: some of the moderately to highly invasive species provide timber and non-timber forest products. These include S.campanulata, L. leucocephala, Syzgium jambos, and Mangifera indica (mango).
Rojas-Sandoval, Presley, and Willig (2026) also analyzed FIA data to assess how non-native tree species affect the biodiversity and composition in three forest types: dry, moist, and wet forests. Unlike Potter et al. (2022), they found that non-native tree species are reshaping native tree assemblages in Puerto Rican forests, leading to significant declines in native species abundance, richness, evenness, and diversity.
The transformation is greatest in the dry forest; there, native richness has declined by more than 90% by some measures. Native communities have become depauperate, dominated by a few species. In subtropical moist forest, native richness peaked at low to moderate invasion levels, then declined. S. campanulata is the dominant non-native species; as noted above, it is found on 41.8% of survey plots in this biome. In subtropical wet forests, native species richness and diversity were highest in uninvaded and lightly invaded plots, followed by marked declines at higher levels of invasion. This is largely driven by that one species, S. campanulata (found on a third of the survey plots in this biome).
The dry forest suffered the greatest proportional loss of biodiversity, including the largest proportional declines in native species richness. Wet forests also experienced strong declines in native richness & abundance. However, since wet forests had much higher initial diversity & structural complexity, their proportional decline in biodiversity is less. Thus, invasion effects differ among forest types depending on initial diversity, resource availability, land-use history, successional stage, and community composition.
Invasion can make individual plots diverge locally through loss of some rare species or gain of different non-native species. If this happens across the study site, the compositional heterogeneity at broader scales is simultaneously reduced. This results in landscape-level biotic homogenization.
Rojas-Sandoval, Presley, and Willig (2026) say homogenization effects are particularly concerning in insular ecosystems, where high endemism and ecological specialization make native biotas especially vulnerable to displacement.
To their surprise, the key driver on Puerto Rico is the increasing abundance of the non-native trees, rather than non-native species richness (Rojas-Sandoval, Presley, and Willig. 2026).
RECOMMENDATIONS
Potteret al. (2022) advise limited efforts to eradicate or control the eight species that occurred only as small stems on a couple of survey plots. These are probably incipient invasives. They name specifically Schinus terebinthifolius (Brazilian pepper) – a species already recognized as moderately invasive in Hawai`i and seriously invasive in peninsular Florida. In 2019 USDA APHIS approved release of two biocontrol insects in Florida targetting Brazilian pepper.
infestation of Brazilian pepper in the Florida Everglades; photo courtesy of Tony Pernas, National Park Service
I recommend that, in order to avoid having to consider importing those biocontrol agents to Puerto Rico, island conservation stakeholders should focus eradication efforts on this species now while it is still – apparently – not widespread.
Rojas-Sandoval, Presley, and Willig (2026) are bolder. They call for implementation of more effective policies to prevent additional introductions and spread of the invasives already on Puerto Rico or nearby islands. They suggest that officials focus on the species named in their dataset. In addition, scientists should also collect data on understory dynamics to get a more comprehensive assessment of bioinvasion in the forest. Rojas-Sandoval et al. (2026) also urge implementation of policies aimed at reducing anthropogenic disturbances in these fragile ecosystems. One component of this program is for those responsible for forest management, conservation, and climate adaptation to incorporate invasion dynamics into their strategies. They remind us that Caribbean islands host extraordinary species richness – many of which are endemic. So protecting these biological riches is of global importance.
Preventing anthropogenic disturbance is likely to aid control of invasive plants. Zimmerman et al. (2021) found that the better-protected forests of the Caribbean National Forest was less invaded by vascular plants than were similar areas that had higher levels of human disturbance. However, this was not the case regarding invasive mammals and some invertebrates. Other than the passing reference to Austropuccinia psidii on Syzygium jambos, none of the studies considered pests or pathogens hosted by trees or other plants.
Other Taxa
Zimmerman et al. (2021) also evaluated invasive animal species. They report that six species of vertebrates are invasive in Caribbean National Forest. Black rats (Rattus rattus), mongoose (Herpestes auropunctatus), and feral cats (Felis catus) are widespread through both disturbed and undisturbed mature forest. Each threatens many native species. The black rat also preys on seeds of several native tree species. House mouse (Mus musculus) is also very common, but restricted to roadside habitats. Cane toad (Rhinella marina) and green iguana (Iguana iguana) are also present. The green iguanas was introduced relatively recently and is rarely observed in CNF. Cane toads have been established much longer. Zimmerman et al. (2021) report no impacts.
Surprisingly, they report no introduced bird or fish species in El Yunque, even the species are common on the island and in parts of the Forest having a history of anthropogenic disturbance.
Two invertebrate bioinvaders are reported as ubiquitous in the National Forest: a hybrid honeybee and Aedes aegypti mosquito. The Africanized honeybee has evolved gentle behaviors and is no longer a great threat to cavity nesting birds, including the endangered Puerto Rico Parrot (Amazona vittata). Two species of introduced earthworms, Pontoscolex corethrurus and Ocnerodrilus occidentalis, are widespread in El Yunque; a third, Drawida barwelli, is found only in lower-elevation forest areas outside NF. The earthworms alter biogeochemical cycling in the soil, which might further influence plant community dynamics. Non-native slugs and snails do not appear to be spreading rapidly or damaging native plant species. Zimmerman, Rojas-Sandoval, and Shiels (2021) warn that additional invertebrates might be of concern in the future, since they can expand rapidly after forest destructions caused by hurricanes.
See also the brief summary of invasive species on Puerto Rico included in the Regional Summary Appendix for the Southeast in Poland et al. (2019). I note mentions of the South American Harrisia cactus mealybug (Hypogeococcus pungens, which is killing columnar cacti in the islands’ dry forests.
SOURCES
Lugo, A.E., J.E. Smith, K.M. Potter, H. Marcano Vega, C.M. Kurtz. 2022. The Contribution of Non-native Tree Species to the Structure and Composition of Forests in the Conterminous United States in Comparison with Tropical Islands in the Pacific and Caribbean. USFS International Institute of Tropical Forestry General Technical Report IITF-54.
Poland, T.M., Patel-Weynand, T., Finch, D., Miniat, C. F., and Lopez, V. (Eds) (2019), Invasive Species in Forests and Grasslands of the United States: A Comprehensive Science Synthesis for the United States Forest Sector. Especially the Appendix on the Southeast and Caribbean. Springer Verlag. Available gratis at https://link.springer.com/book/10.1007/978-3-030-45367-1
Potter K.M., Riitters, K.H. and Guo. Q. 2022. Non-native tree regeneration indicates regional and national risks from current invasions. Frontiers in Forests and Global Change Front. For. Glob. Change 5:966407. doi: 10.3389/ffgc.2022.966407
Rojas-Sandoval, J., R.L. Tremblay, P. Acevedo-Rodriquez, H.D. Soltero. 2017. IAS plant species in the West Indies: geog, ecological and floristic insights. Ecology and Evolution 2017; 1-12
Rojas-Sandoval, J., Presley, S.J. and Willig, M.R. 2026. Increasing non‑native tree abundance reshapes biodiversity and composition of tropical forests. Biol Invasions28, 84 (2026). https://doi.org/10.1007/s10530-026-03802-w
Zimmerman, J.K., J. Rojas-Sandoval, and A.B. Shiels. 2021. IAS in PR: The View From El Yunque. Front. Ecol. Evol. 9:640121. doi: 10.3389/fevo.2021.640121
Posted by Faith Campbell
We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.
For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm
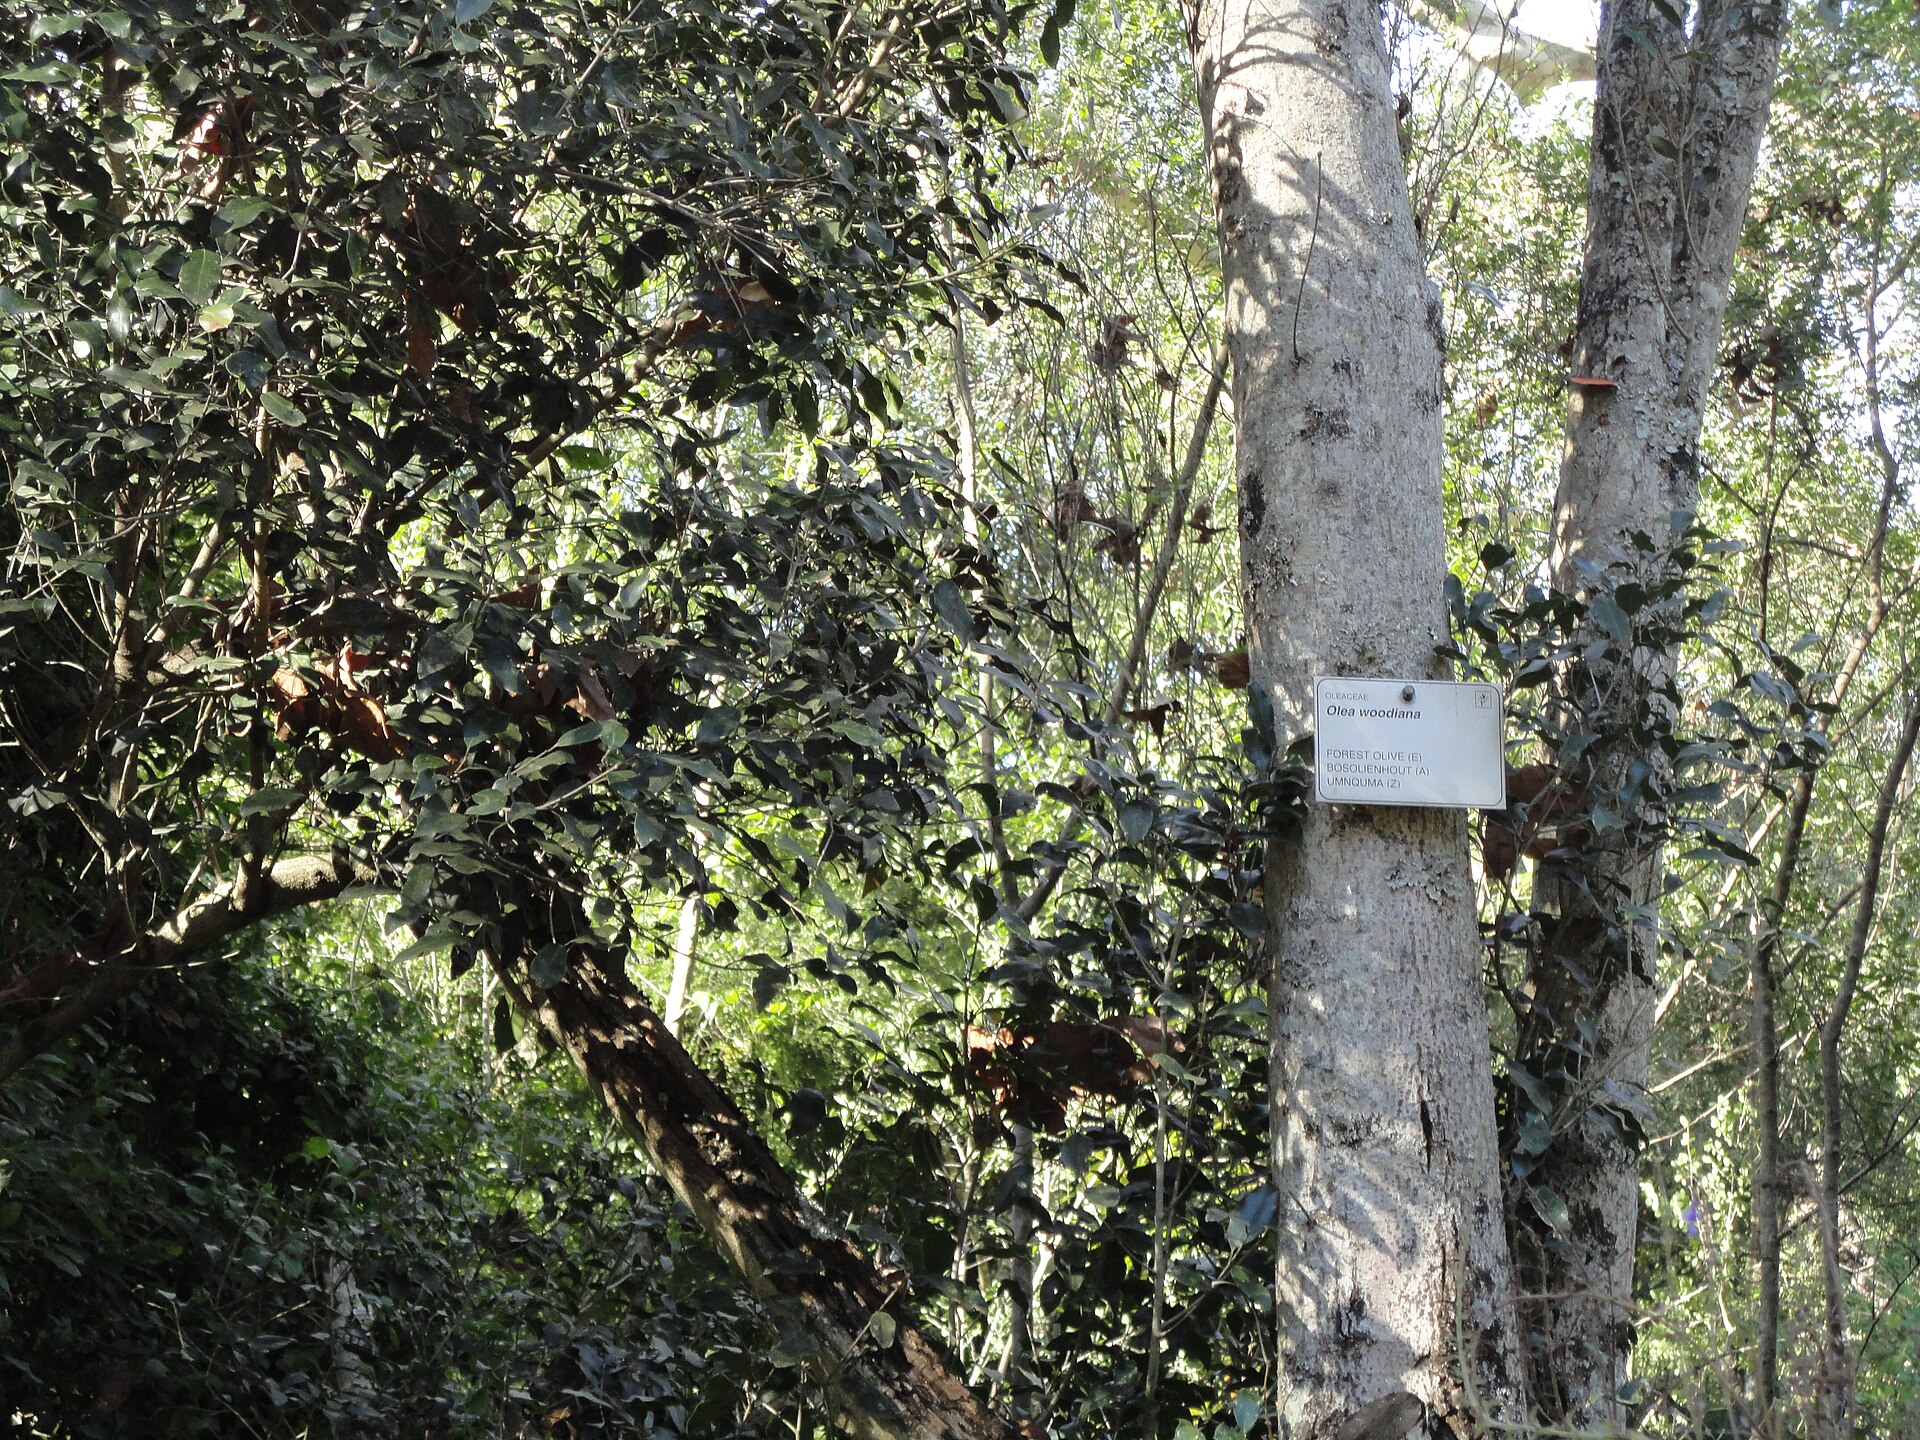
native Olia woodiana in forest of Kwa-Zulu-Natal, South Africa. Photo by MJK via Wikimedia
The forests of the Southern Hemisphere faces an elevated risk from introductions of tree-killing arthropods and pathogens. I have already blogged about individual threats to the trees of South Africa, Australia, South America, and Madagascar. This blog will add information about those invasions and provide an overview and call for action.
Burgess and Winfield (2026) [full citation at the end of this blog] – eminent pathologists from South Africa – warn their colleagues that the economic and biological barriers that have long protected the biomes of the Southern Hemisphere from bioinvasion have now collapsed. While these countries remain geographically distant from each other and the Northern Hemisphere, and their floras are certainly still unique, they are now participating in global trade. In addition, they increasingly rely on industrial plantation forestry dominated by non-native tree species – some of them from the North. Finally, climate change is putting additional stress on all these systems.
Burgess and Winfield (2026) advise their colleagues to learn lessons from the alarming history of bioinvasion in the Northern Hemisphere. Over the past century, these forests have been battered by a series of invasions by tree-killing pathogens. They mention the examples we know too well: chestnut blight (Cryphonectria parasitica), white pine blister rust (Cronartium ribicola), “Dutch” elm disease (Ophiostoma ulmi/Ophiostoma novo-ulmi), pine wilt nematode (Bursaphelenchus xylophilus), sudden oak death (Phytophthora ramorum), ash decline (Hymenoscyphus fraxineus), laurel wilt (Harringtonia lauricolia), ʻōhiʻa or myrtle rust (Austropuccinia psidii), https://www.dontmovefirewood.org/pest_pathogen/ohia-rust-html/ and rapid ʻōhiʻa death (Ceratocycstis lukobia and huliohula). They do not address the similarly depressing history of arthropod interchanges among these realms.
Burgess and Winfield (2026) warn that these invasions are not anomalies but rather predictable outcomes of global commerce – especially in “plants for planting” – interacting with the ecological vulnerability arising from the biogeographic similarity of these temperate and boreal forests. The Northern Hemisphere is dominated by a single flora (the Holarctic).
The Southern Hemisphere has an astounding seven floral kingdoms, distributed as follows: Chile-Patagonian, Neotropical, African, Indo-Malesian, Australian, Novozealandic, and Cape. These regions were formerly part of Gondwanaland. Each has an exceptionally high level of endemism (Burgess and Wingfield 2026), but with phylogenic relationships to the flora of other regions. Changing trade patterns are opening introductory pathways for exchange of tree pests hosted by related but geographically distant species. The regional floras’ uniqueness multiplies the conservation importance of protecting them. I summarize Southern Hemisphere countries’ levels of endemism at the end of this blog.
The lessons Burgess and Wingfield (2026) draw from the bioinvasion history of the Northern Hemsphere include:
1) Trade in living plants – and even seeds – creates a high risk that accompanying microbes will be introduced. As noted by others – e.g., Tanney et al. (2025) – members of each plant species’ “phytobiome” are ubiquitous, diverse, difficult to detect, and sometimes capable of causing serious diseases, especially in naïve hosts.
2) After introduction, these microbes can evolve rapidly to adapt to new environments or hosts. They often become more aggressive and difficult to manage in the process. Plant health officials need to anticipate this evolution.
3) Impacts can be catastrophic when a dominant tree species is killed. When chestnut blight killed the vast majority of chestnut trees in North America it destabilized ecosystems and reshaped successional trajectories.
4) The threat is magnified when the receiving ecosystem is a forestry plantation because of the extensive monocultures.
Building on Burgess and Wingfield (2026) and other sources (where noted), I provide the following summary of threats to native and planted forests in these regions. Some, e.g., Phytophthora cinnamomi and Sirex noctilio, were introduced many decades ago. But too many are recent arrivals.
I. Threats to tree species native to the region.
1) Australia
trees killed by Phytophthora cinnamomi; photo by Western Australia Parks & Wildlife
Carnegie et al. (2026) report that more 300 non-native insect pests, pathogens and nematodes are established on tree or shrub hosts in Australia. Twenty percent have caused moderate to high impacts to commercial plantations, urban forests, or trees in natural ecosystems.
Phytophthora cinnamomi: As noted, this pathogen was introduced decades ago. It has devastated jarrah (Eucalyptus marginata) forests and diverse plant communities. It causes severe mortality in Proteaceae, Epacridaceae, and Fabaceae. Of ~5700 described plant species in the state of Western Australia, 40% ( >2,300) can be killed (Carnegie et al. 2026).
Austropuccinia psidii (myrtle rust): threatens trees in the Myrtaceae worldwide. The rust has spread widely recently, causing severe ecological impacts in invaded regions. The “epidemic strain” introduced to Australia (and other regions) does not infect the commercially important genus Eucalyptus, which probably explains Australian authorities’ lackluster response. However, other lineages of the pathogen found in South America do infect Eucalyptus; introduction of one of these to Australia could be disastrous. Cautionary example of how rapidly a plant pathogen can conquer new ecosystems (Burgess and Wingfield 2026). Already, plant 76 species have been determined to be at risk to myrtle rust. The early focus has been on understory species in the eastern rainforests. Now that myrtle rust has been detected in Western Australia, a biodiversity hotspot with more than a thousand Myrtaceae taxa, most of which are expected to be susceptible. [Summary of Proceedings: Australian Myrtle Rust Conference Sydney, June 2023]
Polyphagous shot hole borerEuwallacea fornicatus s.s. (PSHB) and associated pathogen F.euwallacea were detected in 2021, probably three years after it established in Western Australia. Nearly 9% of hosts are regionally indigenous species, 21.3% native to other parts of the continent. There will probably be a considerable impact on the health of conservation reserves & national parks in the future. After trying for four years to eradicate the population, in November 2025, the National Management Group began a transition to a Management Response Plan. This new approach will impose significant additional expenses on local governments and communities for tree removal and replacement (Dell, Xu, & Chi 2026). Meanwhile, the state of New South Wales (2,000 miles away on the other side of the continent) initiated surveillance for PSHB. An assessment determined that 47% of urban trees in Sydney are susceptible to PSHB (Carnegie et al. 2026).
Erythinagall waspQuadrastichus erythrinae (Carnegie and Nahrung 2019). Although Australia is home to at least one native species in the Erythrina genus, E. vespertilio, this pest has not been included on the environmental pest watch list.
2) New Zealand
native forest on North Island, New Zealand, with kauri tree; photo by F.T. Campbell
Kauri dieback / Phytophthora agathidicida is killing Agathis australis, a keystone species that shapes forest structure and has enormous cultural importance for the Maori.
3) South Africa
Phytophthora cinnamomi — in the country since 1931 — threatens ecosystem collapse in Cape Floral Kingdom (Burgess and Wingfield 2026).
Polyphagous shot hole borerEuwallacea fornicatus s.s. and associated pathogen F.euwallacea The largest outbreak of Fusasrium disease in the world: it is present in every province except Limpopo. The Disease is recorded on 162 tree species. Seventy-eight of these species are indigenous to the country. Eighty-four are “competent” hosts and 78 are “Fusarium colonised” hosts (Townsend, Hill, Hurley and Roets 2025).
Fungus Seiridium neocupressi detected on the native tree, Widdringtonia nodiflora yearThe two other species in the genus, W. wallichii and W. schwartzii, occur in small endemic and threatened populations (Wingfield et al. 2022).
4) Madagascar
Leptographium calophylli killing an endemic tree species in mid-level elevation humid and subhumid forests, Calophyllum paniculatum.
5) South America
Polyphagous shot hole borerEuwallacea fornicatus s.s. and associated pathogen F.euwallacea has been detected in Brazil, Argentina, and Uruguay. Dell, Xu, & Chi (2026) report that in Uruguay a significant number of native species are reproductive hosts for the beetle. Models developed by Coates and Philips (2026) indicate PSHB could thrive in more suitable habitats.
One of the continent’s native conifers, Austrocedrus chilensis is under attack by both an introduced aphid, Cinara cupressi and the pathogen Phytophthora austrocedri
Chilean cypress; photo by LBM via Wikipedia
Lantschner et al. (2026) identified seven independent introduction events of E. fornicatus: to the continental U.S., Hawai`i, South America, Central Europe, Spain, Türkiye, & South Africa.
II. Threats to plantations:
1) Co-evolved insects and pathogens have followed their Pinus hosts to plantations in the Southern Hemisphere due to biosecurity failures
Insects: Sirex noctilio (decades ago); recently Sirex obesusin Brazil (2023); Orthotomicus erosus and Cyrtogenius luteus (Stazione, Soliani, and Cognato 2026).
2) Because the Myrtaceae family is distributed around the Southern Hemisphere, plantations of Eucalyptus trees are now being damaged by both pathogens from their native Australian range (Teratosphaeria spp.) and local pathogens that have switched hosts (Chrysoporthe cubensis and Chrysoporthe deuterocubensis).
Burgess and Wingfield (2026) express fear that another set of pathogens, rapid ohia death (Ceratocystis lukuohia and Ceratocystis huliohia) might spread from Hawai`i farther across Oceania to New Zealand and other locations with important species in the Metrosideros genus. I note that the more virulent (on ʻōhiʻa) C. lukuohia belongs to an Asian-Australian clade (Luiz et al. 2023).
Australia
I blogged in November 2022 about how surprising tardy Australia was in implementing phytosanitary programs to protect the nation’s forests. Scientists had spent 30 years trying to get such a program implemented. Burgess and Wingfield (2026) point out that 16 of 17 pathogens detected in Australia over the period 1996 – 2017 had established; several had had major impacts. None has been eradicated. They also note that the introduction of Austropuccinia psidii exposed significant weaknesses in post-border surveillance and response.
The Australian federal govt has implemented a detection trapping program targeting the Asian spongy moth (= flighted spongy moth complex) at the 4 major ports (i.e., Melbourne, Hastings, Geelong and Portland) since 1996.
Carnegie et al. (2026) describe some helpful steps. They focus on establishment in 2022 of a National Forest Pest Surveillance Program (now called Forest Watch Australia). The program is funded by a levy on forest plantation growers and State governments, based on the relative risk to each region. Surveillance efforts are concentrated in areas deemed high risk areas for entry and establishment of forest pests. Program is coordinated through the federal agency, Plant Health Australia. It provides professional training for surveillance and diagnostic staff on an annual basis. Staff also conduct risk modelling and analysis to identify high-risk areas for surveillance in all major capital cities — Sydney, Melbourne, Brisbane, Hobart, Adelaide, Perth and Darwin.
The Australian program encounters the universal challenges regarding sustained resources, the diagnostic burden placed on scientists, and ownership of data. Carnegie et al. (2026) and Burgess and Wingfield (2026) discuss the growing availability of new tools for detection, e.g., molecular diagnostic tools.
Response options are guided by the national Emergency Plant Pest Response Deed and PlantPlan, which outlines agreed government and industry responsibilities and cost-sharing protocols.
Carnegie et al. (2026) praise especially the sentinel tree component of the surveillance program. Participants include governments at the federal, state, and municipal levels; botanical gardens; and industry. In 2024/25, trained staff inspected 5,136 trees of more than 50 species across 45 genera nationwide. Thanks to this expanded effort, the detection rate of new species has doubled since 2018, from ~ 1.5 to ~ 3 / year. Still, in three of four cases discussed by Carnegie et al. (2026), the introduced organisms were determined to be too widespread for eradication to be successful. They cite the PSHB outbreak in Perth as an example. Carnegie et al. (2026) advocate strengthening sentinel tree surveillance in urban landscapes so detection will occur sufficiently early to allow consideration of initiating an eradication or containment response. One worrisome aspect: there is no requirement to conduct more thorough surveillance or diagnostics on a species detected in the country once it has been ruled not “of concern”.
Burgess and Wingfield (2026) advocate embracing broader preventative approaches that address the underlying mechanisms of pathogen emergence and spread. I forthcoming blog will discuss proposed new approaches.
Background: Southern Hemisphere Flora
South Africa
As I blogged recently, South Africa’s flora is diverse (more than 20,000 indigenous species) and has high levels of endemism. That blog did not discuss the Myrtaceae family – my focus now because of the spread of the pathogen Austropuccinia psidii. According to Braam van Wyk and Hugh Glen (pers. comm.), the country has 24 native Myrtaceous species. These include 14 species in the Eugenia genus, six in the Syzygium genus. The one Metrosideros grows in the Cape Floristic Region. All the others occur in forest or grassland along the Indian Ocean Coastline well into Mozambique and further inland – some into Botswana and Zimbabwe.
Australia
Australia ranks second on Earth in the proportion of its flora that is endemic: 88% of plants. Australia comprises the native range of 38% of all Myrtaceae species on Earth, and of 66% of genera in the family (Brett Summerell, 2023 workshop). These 87 or 88 genera contain ~ 2,250 species and subspecies (Makinson 2018). This plant family constitutes ~10% of the continent’s native flora. They occur in 11 of 13 major vegetation formations (Carnegie et al.2026). The southwestern corner of Western Australia alone has ~5700 described plant species (Carnegie et al 2026).
Rhodomyrtus psidioides – one of the Australian Myrtaceae under greatest threat from myrtle rust; photo by Zaadero via Wikimedia
The island of Madagascaris home to 12,000 plant species, of which 83% are endemic.
SOURCES
Burgess T.K., and M.J. Wingfield. 2026. Unveiling a Hidden Menace: Invasive Tree Pathogens, Less Known but Increasingly Threatening Southern Hemisphere Forests Annual Review of Phytopathology #s
Carnegie AJ, Summerell BA, Trollip C, Tovar F, Smith DI and McDonald J (2026) Sentinel trees for early detection of non-native forest pests and pathogens in AU. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183
Ceriani-Nakamurakare, E., Johnson, A.J. and Gomez, D.F. (2023) Uncharted Territories: First report of Euwallacea fornicatus (Eichhoff) in South America with new reproductive hosts records. Zootaxa, 5325 (2), 289–297. https://doi.org/10.11646/zootaxa.5325.2.10
Lantschner, M.V., Ceriani-Nakamurakare, E., Johnson, A.J. et al. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis, two global emerging pests. J Pest Sci99, 100 (2026). https://doi.org/10.1007/s10340-026-02070-w
Luiz, B.C., C.P. Giardina, L.M. Keith, D.F. Jacobs, R.A. Sniezko, M.A. Hughes, J.B. Friday, P. Cannon, R. Hauff, K. Francisco, M.M. Chau, N. Dudley, A. Yeh, G. Asner, R.E. Martin, R. Perroy, B.J. Tucker, A. Evangelista, V. Fernandez, C. Martins-Keli’iho.omalu, K. Santos, R. Ohara. 2023. A framework for establishlishing a rapid ‘Ohi‘a death resistance program New Forests54, 637–660. https://doi.org/10.1007/s11056-021-09896-5
Stazione, L., Soliani, C., Cognato, A. et al. Reconstructing the invasion history of the bark beetles Orthotomicus erosus and Cyrtogenius luteus (Coleoptera, Curculionidae, Scolytinae) in South America. Biol Invasions28, 49 (2026). https://doi.org/10.1007/s10530-026-03779-6
Tanney, J.B., M. Kemler, M. Vivas, M.J. Wingfield, and B. Slippers. 2025. Silent invaders: the hidden threat of asymptomatic phytobiomes to forest security. New Phytologist (2025) 247: 533–545 doi: 10.1111/nph.70209
Wingfield, M.J. S. Marincowitz, N.Q. Pham, F. Roets, T. Paap, B.D. Wingfield, J. Aylward. 2022. Cypress canker: An important disease discovered for the first time on a native South African tree. Plant Pathology 2022;71:1735-1742
Posted by Faith Campbell
We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.
For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm