New Zealand prepares – but perhaps not sufficiently

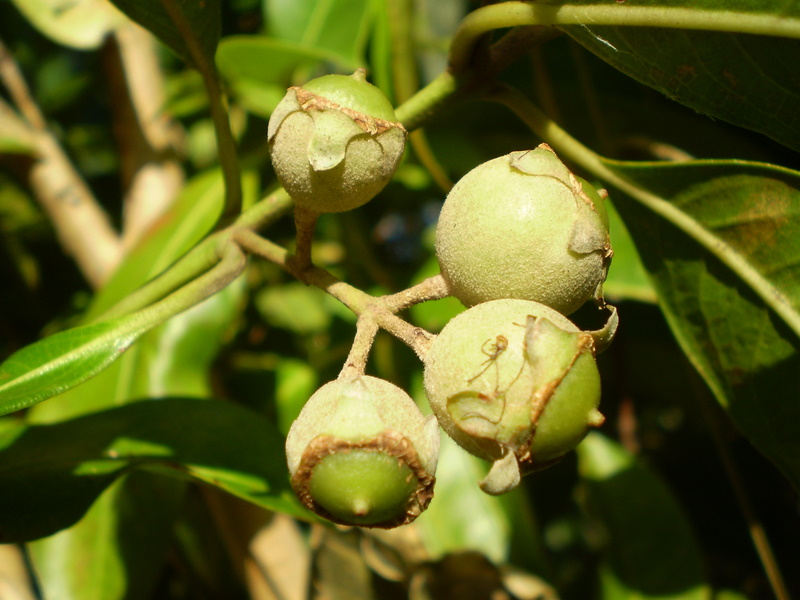
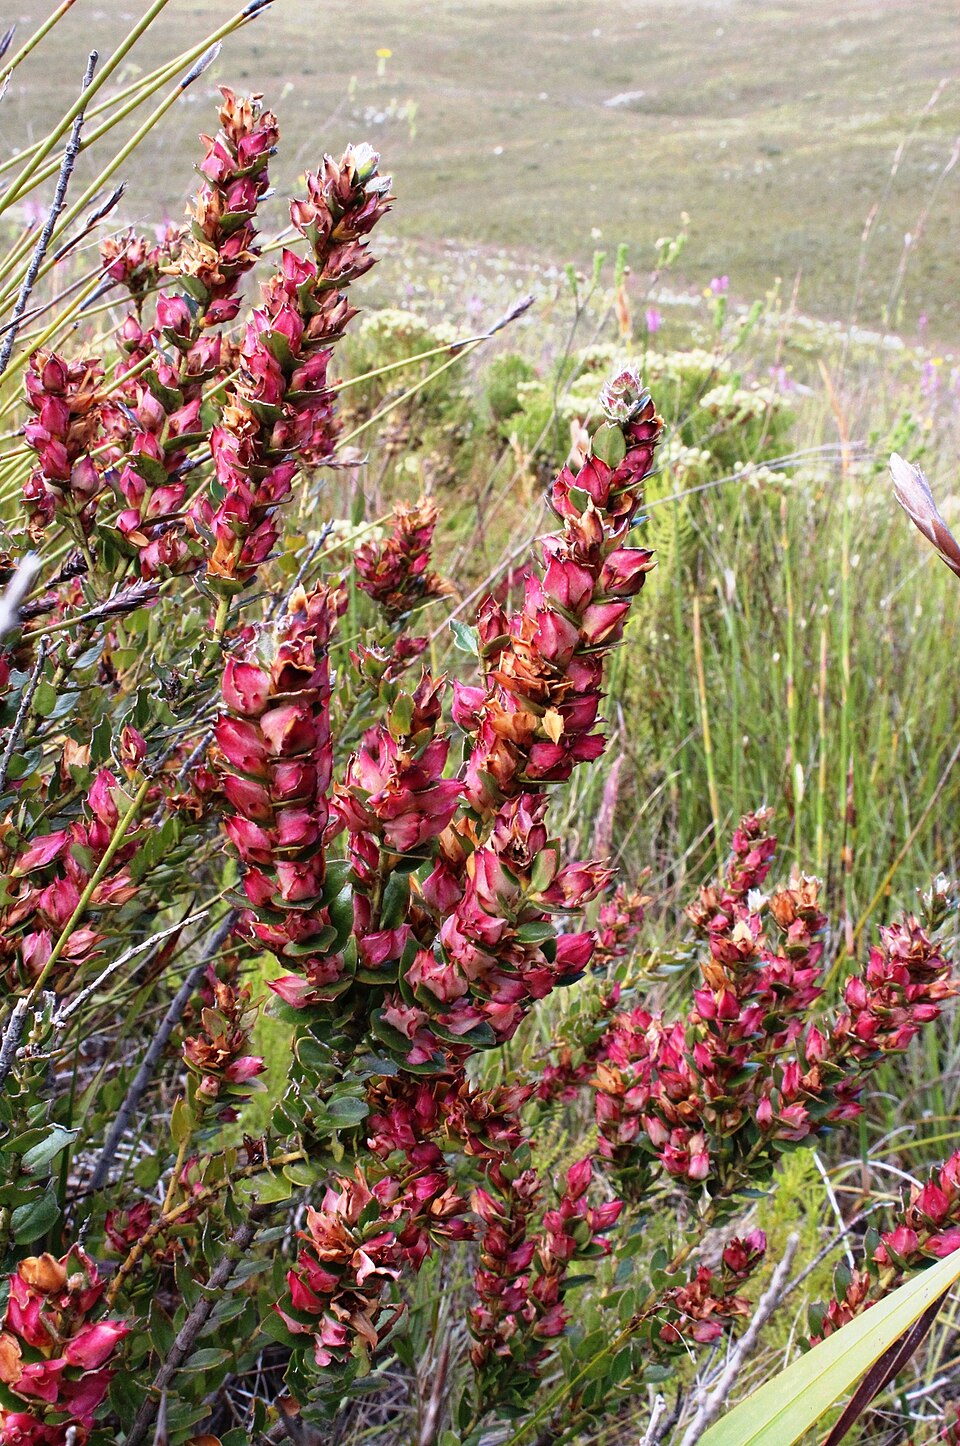
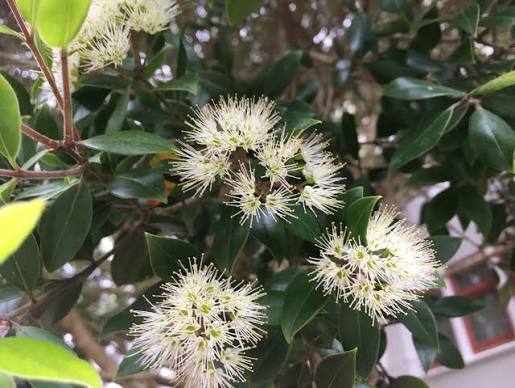
Metrosideros bartlettii; photo by Bodleye1 via Wikimedia Media

I rejoice that New Zealanders are exploring the risk to Aotearoa New Zealand and South Pacific islands posed by the rapid ‘ōhi‘a death (ROD) pathogens, Ceratocystis lukuohia and C. huliohia. See Marroni et al., – full citation at the end of this blog.

Marroni et al. (2026) note that several species in the genus Ceratocystis cause severe disease in native and cultivated plants following their introduction to new regions. Several of the more than 40 species in the genus have demonstrated a capacity to infect a wide range of hosts and, in some cases, to attack new hosts in novel regions.

The stakes are high. These islands are home to 54 of the 58 species in the Metrosideros genus – the genus of Hawaii’s ‘ōhi‘a lehua trees (Metrosideros polymorpha) – an endemic species of immense ecological and cultural importance. Aotearoa New Zealand alone has 12 native Metrosideros species. Four of these species are already under conservation threat. Only 31 Bartlett’s rātā (M. bartlettii) trees remain in the wild. Another species, pōhutukawa(M. excelsa), has declined 90% in abundance since Polynesian and European settlements — although it is not formally listed as threatened. (Why not?) Trees on other South Pacific islands are also apparently at risk. Metrosideros collina is widespread on these islands and is known to be susceptible to C. lukuohia. Its close relationship to both Hawaiian species and several species on the other islands suggests that related taxa across the region might also be vulnerable.
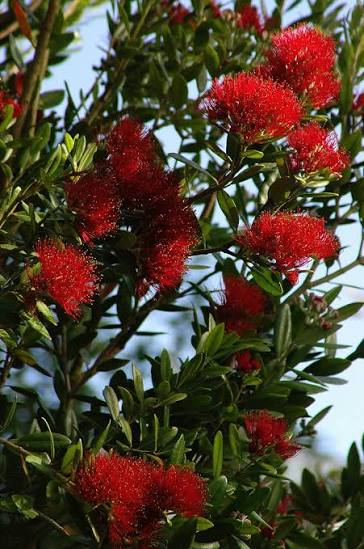
Metrosideros excelsa; photo by Ceili & Roger via Flickr

Marroni et al. (2026) worry that non-Metrosideros species (native or introduced) could also be at risk. They cite the recent finding on Kaua‘i of C. lukuohia in dead camphor trees(Cinnamomum camphora) and death of 60–100% of kiwifruit (Actinidia chinensis) in laboratory tests. So far, coffee, avocado, macadamia, mānuka (Leptospermum scoparium), and two species invasive in Hawai`i, rose apple (Syzygium jambos) and strawberry guava (Psidium cattleianum) have proved not susceptible to C. lukuohia in laboratory tests.

I applaud the New Zealanders for initiating tests of these species’ vulnerability. Preliminary results indicate that M. excelsa might be less susceptible to C. lukuohia than the Hawaiian species. M. perforata (white rātā) and M. fulgens (climbing rātā) have been found susceptible to C. lukuohia.  Pathogenicity tests are under way on additional New Zealand Metrosideros species. Marroni et al. (2026) call for screening of all Metrosideros species. They also suggest that New Zealand plant species – not just Metrosideros spp. – growing in botanical gardens or amenity plantings in Hawai’i should be monitored – application of the “sentinel tree” concept.

The scientists are also evaluating climatic factors. Although most Ceratocystis spp., including the two ROD species, are found primarily in tropical regions, some species cause disease across a broader climatic range. Models indicate that some parts of North Island are suitable now for ROD establishment. Several of the vulnerable species [M. excelsa, M. robusta (northern rātā), M. bartlettii and M. umbellata (southern rātā)] grow on that island. Low winter temperatures appear to preclude establishment on South Island at present. However, rising temperatures associated with global warming is expected to greatly expand ROD’s potential distribution to include nearly all of North Island and most of the South Island (see Figures 1a and 1b in the article). Marroni et al. (2026) say that changes in precipitation – extremely important in disease establishment – are more difficult to model. Many South Pacific Islands probably provide highly suitable climatic conditions year-round.

Worrying Conclusions About Risk

While I admire the New Zealanders’ efforts to prepare, I worry that Marroni et al. (2026)’s conclusions about the level of introduction risk are too optimistic. I fear they put too much faith in the country’s strong phytosanitary policies.

The most likely pathways of introduction are movement of infected plants, their wood, or associated soil or insects. These vectors might be moved during trade or carried by tourists.

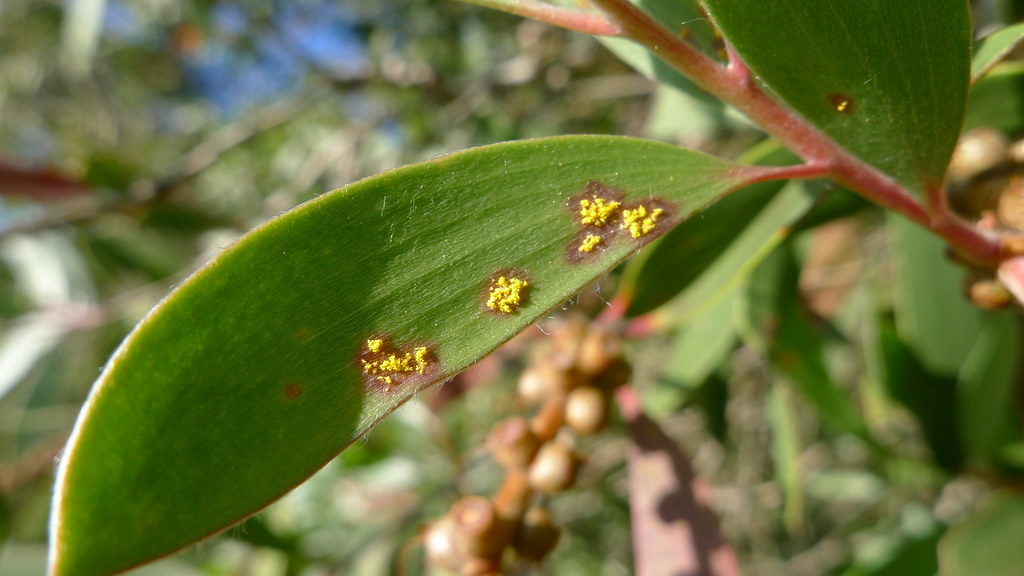
The New Zealand Ministry for Primary Industries (MPI) applies tight requirements on imports of all nursery stock of known Ceratocystis host plants (prompted by a desire to mitigate the risk of introducing the C. fimbriata sensu lato complex). These plants must be inspected both before export and at the port of entry – including testing for the presence of a pathogen and – when indicated — treatment and/or quarantine. Any intercepted putative Ceratocystis species is subject to further diagnostic testing, and infected material is either destroyed or managed according to MPI protocols. Since 2010 New Zealand has prohibited importation of whole plants and cuttings of myrtaceous species (including the Metrosideros genus) from Australia because of the presence of Austropuccinia psidii, causal agent of myrtle rust disease. New Zealand does allow import of tissue culture plantlets from Australia, India, and the United States. Given these stringent phytosanitary requirements and the absence of plant material imported from Hawai`i, Marroni et al. (2026) concluded that the risk of introducing the two ROD pathogens is “low”.

Movement of wood could transport aleurioconidia of C. lukuohia and C. huliohia – thick-walled asexual spores that can survive in infected ‘ōhi‘a wood for at least 12 months. So all wood products derived from infected trees, including logs, timber, firewood, chips, shavings, sawdust, and other wood particles can potentially carry the pathogens. Importation of wood products is managed under seven different standards. New Zealand imports wood products primarily from North America, Southeast Asia, Pacific Islands, and Australia. Marroni et al. (2026) report that various Ceratocystis spp. have been detected on timber originating from South Pacific and Asia multiple times.
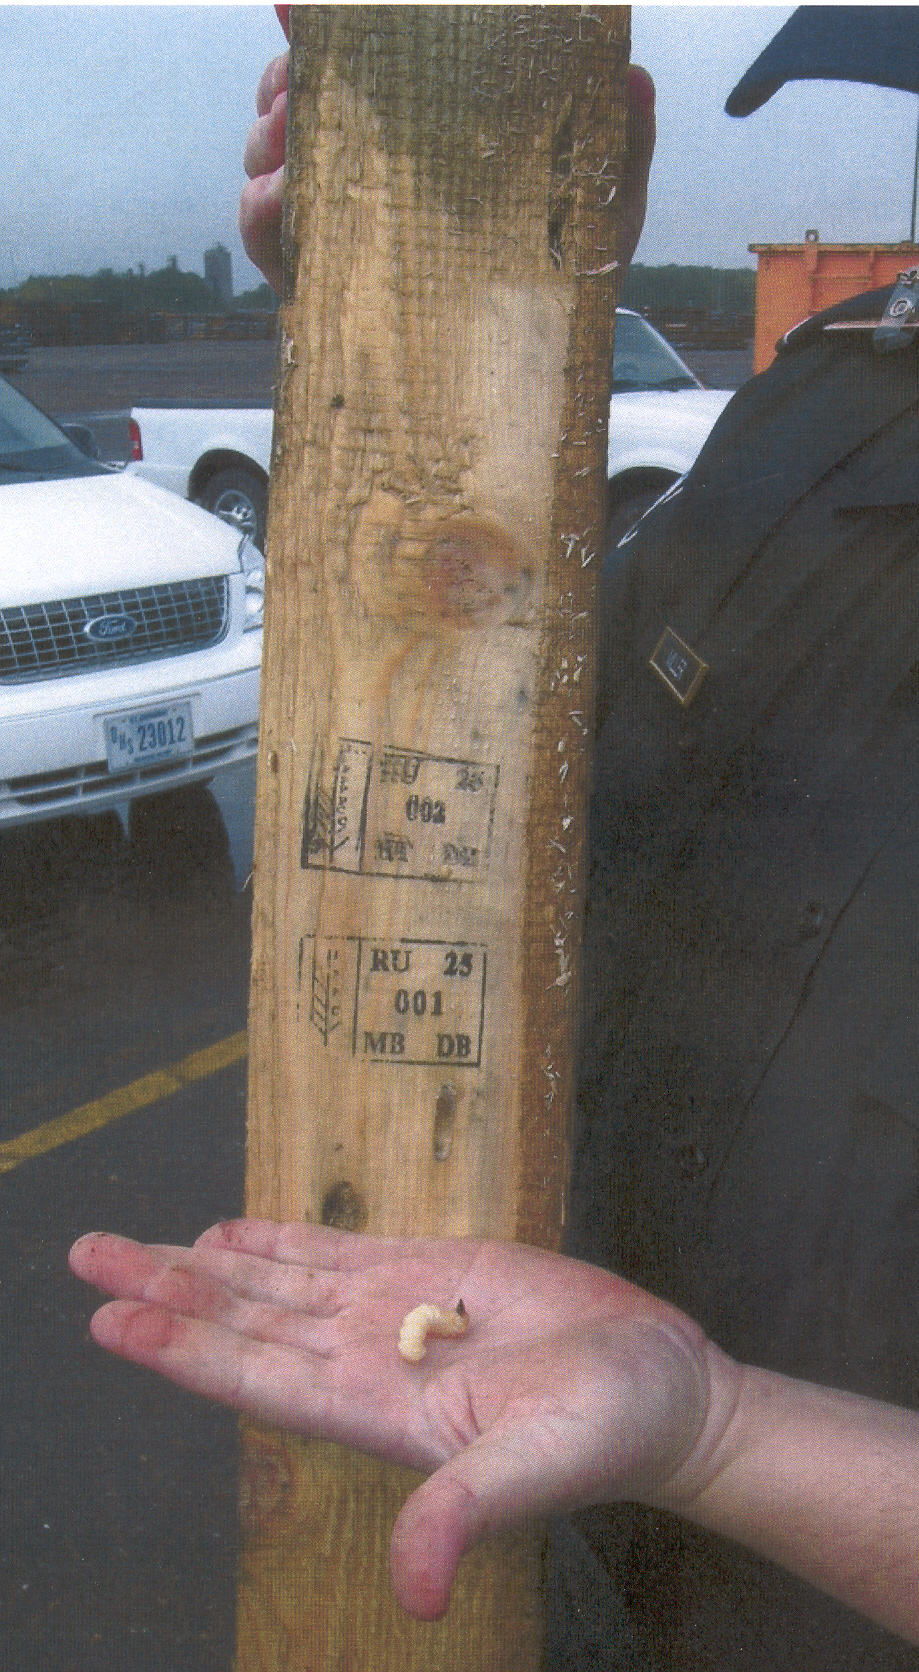
Another type of wood imports is wood packaging material – crates, pallets, spools for cable, etc. Marroni et al. (2026) call the treatments prescribed by ISPM#15 – debarking, heat treatment or fumigation – highly effective in eliminating woodborne pathogens. There have been no detections of Ceratocystis spp. on ISPM#15-compliant SWPM entering New Zealand. Consequently, Marroni et al. (2026) consider the risk of introduction via this pathway to be “low”.

Marroni et al. (2026) do express concern that ambrosia beetles could be introduced via trade in nearly any form. In Hawai`i, the beetles’ frass (wood particles, faeces and beetle fragments) is considered to be a major pathway for spread of the ROD pathogens. Frass can be carried considerable distances on the wind during storms. The frass can also be moved on tools, machinery or footwear.

The New Zealand Ministry for Primary Industries (MPI) prohibits importation of soil; this is enforced by inspection of incoming goods, machinery, containers, and visitors’ footware. They note that despite these measures, accidental intro of soil is still possible, especially via used agricultural machinery and vehicles. One study found soil contamination on 93% of sea containers and flat-rack containers arriving from several Pacific nations. This soil contained viable plant material, plant pathogens, and invertebrates.

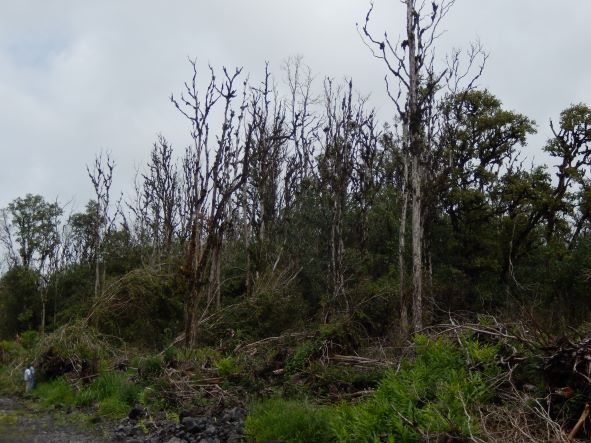
Large numbers of New Zealanders and other Pacific Islanders visit Hawai`i. They could carry ROD propagules back to their home islands in soil on contaminated footwear, clothing, camping equipment, etc. NZ inspectors have found high incidences, counts and diversities of viable bacteria, fungi, nematodes, seeds, and several arthropods on footwear of arriving aircraft passengers. Although Marroni et al. (2026) to not explore this topic in detail, National Park Service and botanical garden websites reveal that ROD is present at several of the sites very popular with tourists. These include Kīlauea, Kīpukapuaulu, the ʻŌlaʻa rainforest, Thurston lava tube, and lower-elevation sections of the Kahuku unit of Hawaii Volcanoes National Park; the Hawaii Tropical Botanical Garden on the Big Island; and Limahuli Garden on Kauai. Overall, the authors consider the risk of introduction by this pathway to be “moderate”.
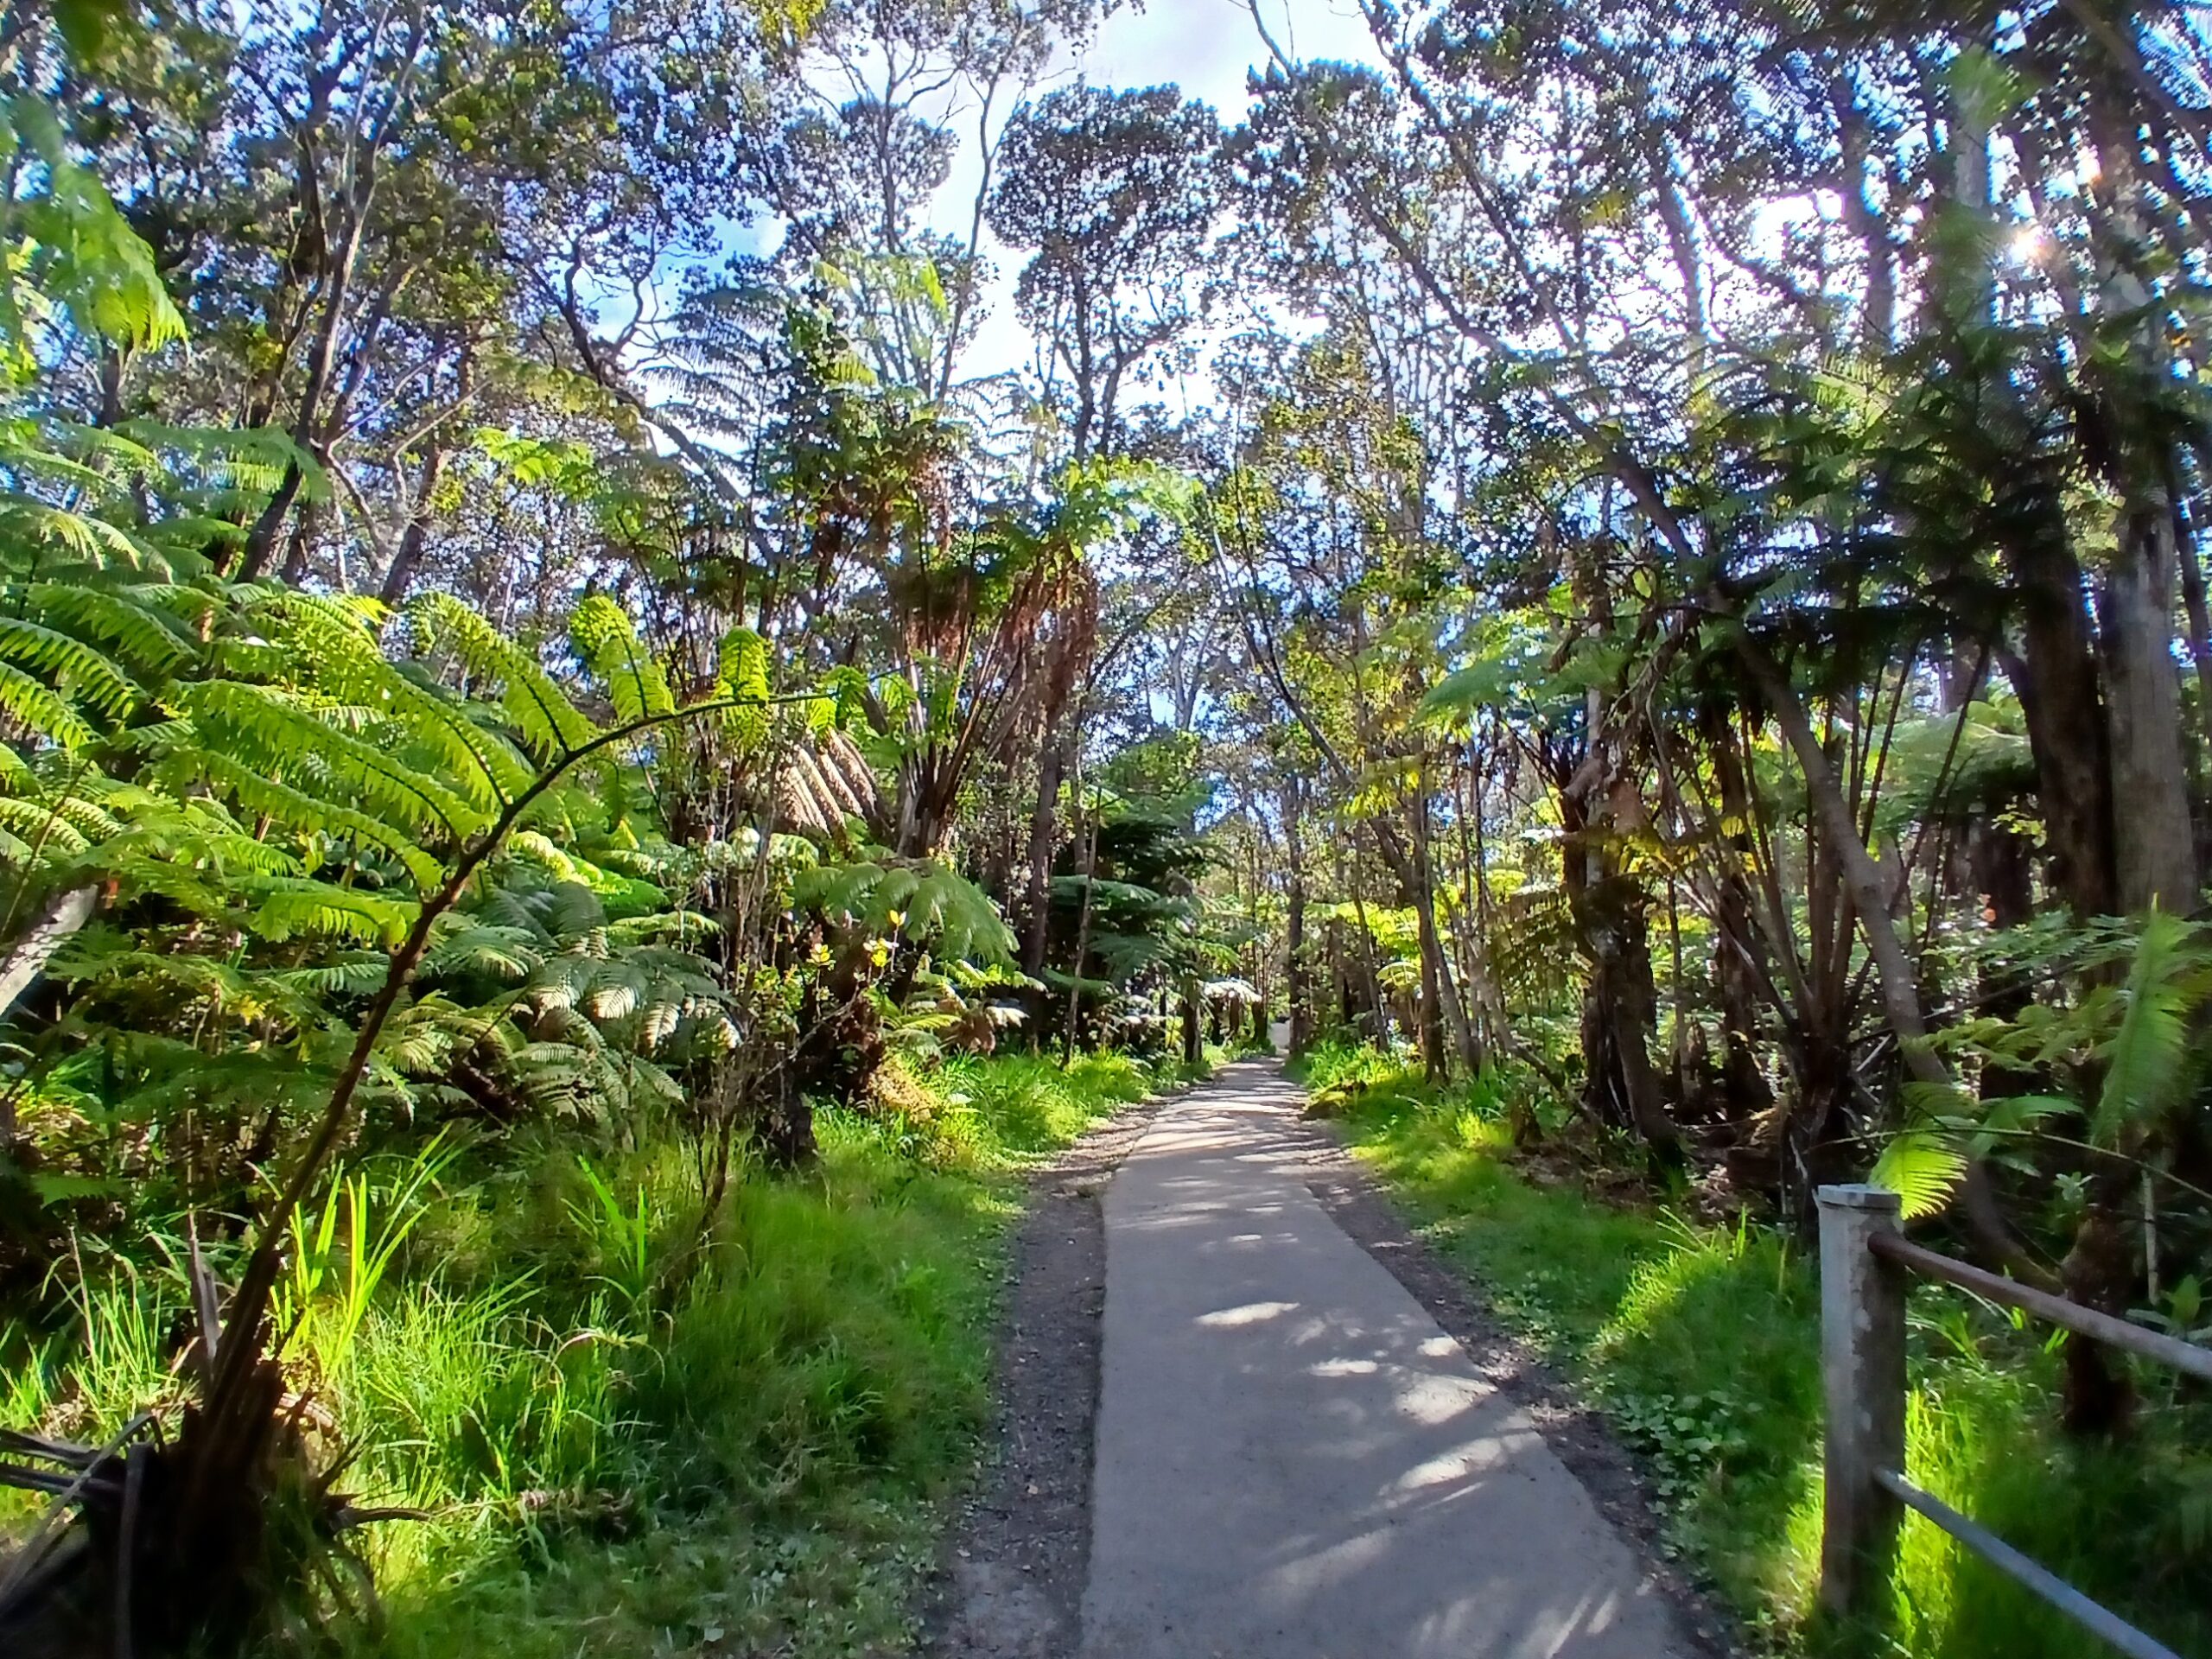
‘ohi‘a trees above trail to Thurston lava tube, Hawai`i Volcanoes National Park; photo by F.T. Campbell

If Ceratocystis lukuohia and C. huliohia were introduced to Aotearoa New Zealand or South Pacific islands, the risk of spread throughout the region seems high. There is the high volume of people and goods – including vehicles – moving among the islands. Wind storms might carry infected frass or insects from one island to another (Austropuccidia psidii is thought to have been introduced to New Zealand from Australia on prevailing winds). All these islands have feral and domestic mammals whose rooting and trampling can wound the trees, exposing them to infection by the pathogen. In New Zealand this risk is greatly exacerbated by the damage caused by the invasive Australian common brushtail possum (Trichosurus vulpecula), which feeds on tree buds and foliage and incidentally strips the bark and breaks branches.

My Concerns

  • Marroni et al. (2026) pay very little attention to the risk of introduction from the native habitats of Ceratocystis lukuohia and C. huliohia. They focus on imports and visitors from Hawai`i. These imports are dominated by aircraft and aircraft parts, scrap metals, gas turbines, seafood and beverages. The imports of primary agricultural or forestry products are in lower volumes. No nursery stock comes from the Islands.

But the Hawaiian outbreaks are caused by introduced pathogens.The native range of the species more virulent in Hawai`i, C. lukuohia, is in Latin America. The native range of C. huliohia is in Australasia! I wish Marroni et al. (2026) had explored the volume and type of imports from these regions.

  • As readers of this blog know, I do not share Marroni et al.’s (2026) sanguine evaluation of the efficacy of ISPM#15 in preventing introduction of wood-boring insects or – especially – fungal pathogens. See this blog describing the impact of polyphagous shot hole borer in one of many places where it has been introduced – perhaps via wood packaging. Or visit other blogs describing continuing failures of the standard by scrolling below “Comments” and “Archive” to “Categories” and click on “wood packaging”.
  • Most host vulnerability testing has focused on vulnerability to C. lukuohia. While C. huliohia is less virulent on Hawaii’s ‘ōhi‘a trees (Metrosideros polymorpha), I think it is unwise to assume that it will behave similarly on naïve tree species on New Zealand or other Pacific islands.
  • Marroni et al.’s (2026) do not acknowledge the difficulties in detecting pathogens on imported plants. See previous blogs describing continuing introductions of pathogens on plan imports by scrolling below “Comments” and “Archive” to “Categories” and click on “forest health” or “plants as vectors”. Perhaps the New Zealand procedures are sufficiently robust to overcome weaknesses detected in the U.S. and elsewhere … but that is not clear.
  • New Zealand scientist do not know how the oomycete Phytophthora agathidicida which kills the endemic kauri tree, Agathis australis was introduced. Does this situation conceal some other pathway?
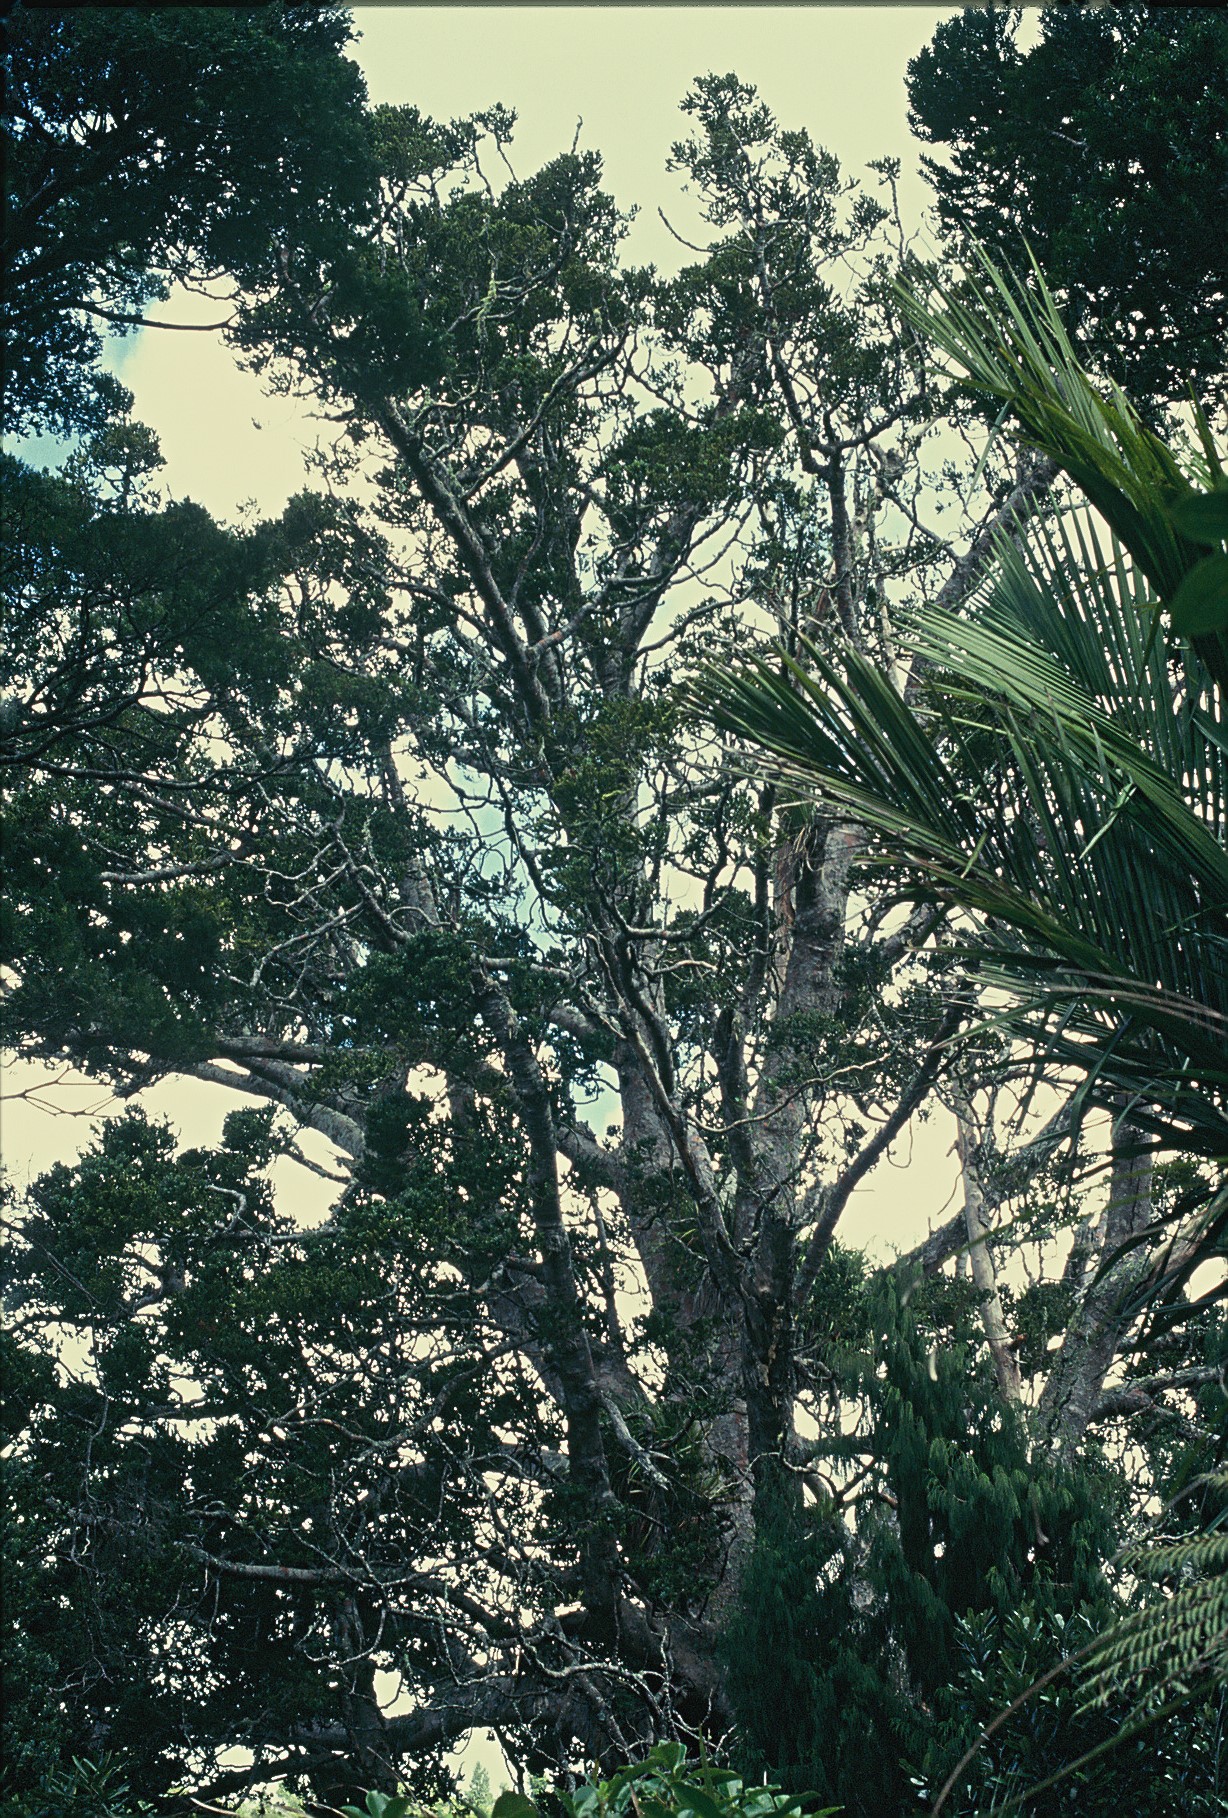
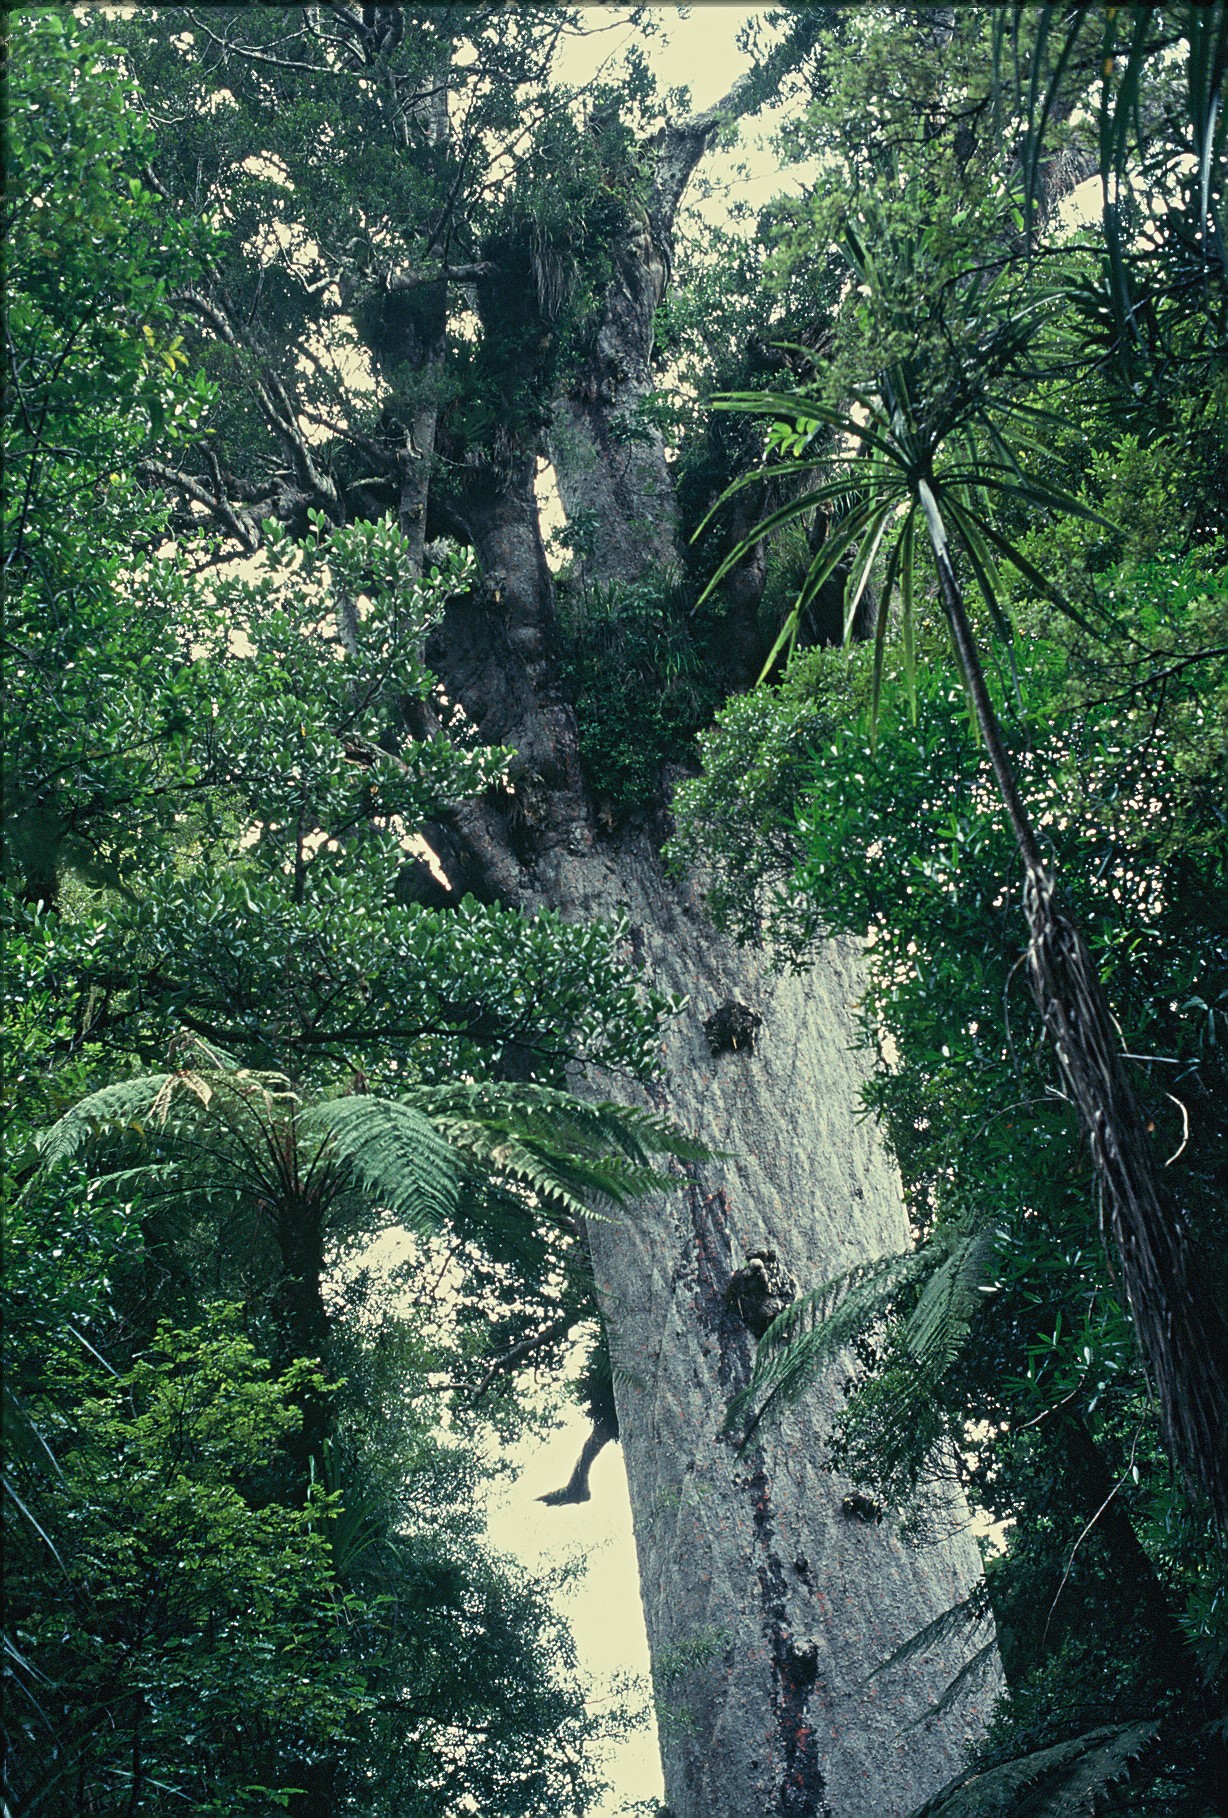
a kauri tree; photo by F.T. Campbell

Uncertainties acknowledged by Marroni et al. (2026)

  • Hawai`i adopting regulations in 2016 to prohibit movement of M. polymorpha plant material from infected regions; this was six years after the disease was first detected. The disease was detected on Kaua‘i in 2018 and 2019, later on Maui and O‘ahu. Do these outbreaks demonstrate the limits of regulation? Or were these outbreaks initiated before the regulation was implemented—given the frequent lag in detection?
  • Asymptomatic infections have been detected on M. excels. Might other species also harbor undetected disease?
  • Scientists don’t know which species of Metrosideros trees, ambrosia beetles, or Ceratocystis fungi are established on which Pacific islands? Their presence or absence is relevant to the possibility of step-by-step spread of the pathogens.
  • Scientists don’t know how the pathogen might respond to seasonal temperature variations on New Zealand.
  • There is very little information on whether tissue culture plantlets can transmit Ceratocystis spp.
  • New Zealand has 12 native and 12 introduced species of Scolytinae, including Xyl. saxesenii [which has transmitted C. lukuohia and C. huliohia under lab conditions]; and Amasa truncata, an Australian ambrosia beetle species implicated in mortality of trees. There is little data regarding which insects associate with Metrosideros.

  • Proposed solutions

Marroni et al. (2026) say New Zealand’s recent sobering experience with myrtle rust https://www.dontmovefirewood.org/pest_pathogen/ohia-rust-html/ demonstrates the importance of quick action if a pathogen is introduced. Suggested priorities are to strengthen pathway management, improve surveillance in climatically suitable regions and at high-risk entry points, and research to address major knowledge gaps relating to host range, climate suitability, potential vectors, and dispersal. Scientists should test a broader range of possible hosts, including representative native forest species and economically important fruit and commercial forestry crops. Other studies are needed to determine which ambrosia beetle species utilize Metrosideros trees.

Pathologists should clarify which Ceratocystis species are already present in New Zealand and the South Pacific. Currently, only Ceratocystis fimbriata sensu stricto is recognized as occurring in New Zealand. However, New Zealand shares many fungi from other taxonomic groups with native forests in Asia and Australia, so Marroni et al. (2026) expect that some Ceratocystis species in the Austroasian clade might also occur naturally in New Zealand without causing obvious disease symptoms. Research is also needed to illuminate the influence of seasonality and local microclimates on disease outbreaks. A better understanding of these variables will inform long-term biosecurity and forest health planning.

Marroni et al. (2026) note that protecting Aotearoa New Zealand forests and primary industries requires collaboration of researchers, biosecurity agencies, Māori and Pacific local communities, and policymakers. They advocate a multidisciplinary approach that considers biological, cultural, and social factors.
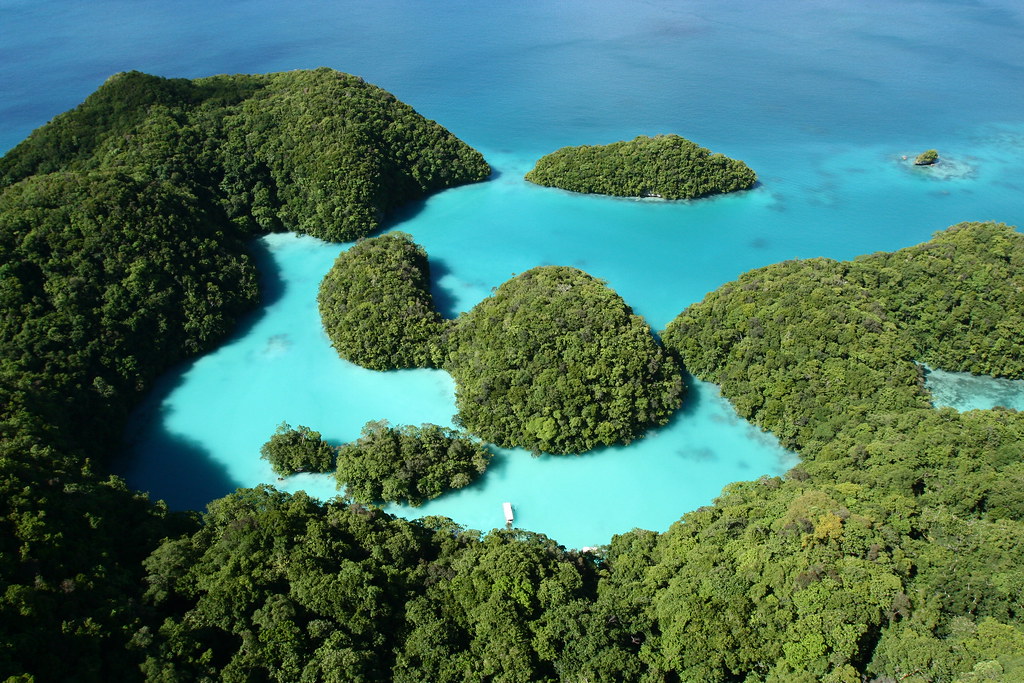
Palau islands; photo by Luka Peternal via Wikimedia

Tree Mortality on Palau

Fear of spread of tree-killing Ceratocystis species across Pacific Island groups is not theoretical. In late 2021 people noticed extensive mortality of mature udeuid (Manilkara udoido) trees in Palau, an independent country in the Micronesian Islands east of the Philippines – so in the North Pacific. Udeuid is a culturally and ecologically important forest tree endemic to just one of the Palauan islands, the largest, Babeldaob Island (Johnson et al. 2025).

Losses exceeded 50% in several areas within the species’ core range. Koch’s Postulates determined the causal agent to be Ceratocystis manginecans, a Brazilian species associated with major disease outbreaks in Asia and elsewhere. Extensive damage to large udeuid trees caused by Typhoon Surigae in April 2021 might have contributed to the outbreak by creating wounds for infection. Four years after the initial detection trees continue to die. This is the first report of C. manginecans on the genus Manilkara andits first detection in the Pacific Islands. Johnson et al. (2025) conclude that C. manginecans poses a serious threat to native forests and cultivated crops in Oceania.

SOURCES

Johnson,J.A., M.A. Hughes,P.I. Bennett,O. Sadang,  K. Roy,  D.R. Kroese,  P.G. Cannon,  N.B. Klopfenstein,T. C. Harrington, and Mee-Sook Kim. 2025. First Report of Ceratocystis manginecans Causing Udeuid (Manilkara udoido) Wilt in Palau Plant Disease December 2025  https://doi.org/10.1094/PDIS-07-25- 1554-PDN 2025

Marroni, M.V., M.R. McNeill, R.E. Campbell, P.R. Johnston, T. Waiariki, A. Puketapu, W. Awarau‑Morris, J. L. Hasna, B. S. Beresford, J. Tyson, B. Weir, G.R. Smith, M. Padamsee, J.K. McCarthy, T.R. Etherington, B. Ganley, B.C. Luiz, L.M. Keith. 2026. The risk of rapid ‘ōhi‘a death to Aotearoa New Zealand and South Pacific. Biol Invasions (2026) 28:207 https://doi.org/10.1007/s10530-026-03896-2

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

EAB detected in Washington State; Pacific Coast states taking action

A newsletter issued by the Oregon Department of Forestry reports lots of action in Oregon and Washington in response to the presence of emerald ash borer (EAB; Agrilus planipennis). (To subscribe to the newsletter, email Jim Gersbach at jim.gersbach@odf.oregon.gov)

Ash-dominated swamp in the Willamette Valley; photo by Wyatt Williams, Oregon Department of Forestry

In Oregon, where EAB was detected in 2022, cities are taking protective actions. In Portland EAB was officially detected inside city limits in late summer 2025 east of the I-205 freeway. So far the beetle has not been reported from elsewhere inside city limits. To better establish where EAB is present, officials plan to girdle 4 ash trees in spring 2027 in hopes that female EAB will be attracted to them and oviposit. Those trees will be cut down in the fall, then examined to determine if any larvae are inside. This method has been used to help pinpoint where EAB is spreading before obvious signs of tree dieback are apparent. Oregon Department of Forestry will demonstrate the techniques for staff from the City of Portland, Oregon Dept. of Agriculture, U.S. Forest Service, Washington Dept. of Natural Resources, and Clackamas Soil & Water Conservation District.

EAB was confirmed within the city limits of Beaverton during summer 2026. The Beaverton City Council has adopted legislation expanding pesticide protection to1,400 ash street treesabove the 600 already treated in 2025. Treatment – injection of emamectin benzoate – is scheduled to begin in spring 2027 and be completed by September 2027. Last year city workers also protected 22 significant native Oregon ash trees (Fraxinus latifolia) over 20” dbh in a city-maintained natural grove that is predominantly ash.

EAB was detected in Silverton by a local tree care professional in summer 2026. The nearby Oregon Garden responded by treating eight ash trees on its grounds – all exotic to the region (seven white ash [eastern North America] & one narrow-leaved ash [Europe]). The Garden receives ~100,000 visitors a year.  The treatments were supervised by Oregon Dept. of Forestry & Oregon Forestry Resource Institute staff.

In Washington State, where EAB was detected in August 2026, near Vancouver, the state has regulated firewood imported from sources outside the state. The quarantine on untreated firewood from outside the state was adopted in February by the state Legislature. It took effect on August 18.  The rule prohibits importation into WA of untreated firewood from outside the state. Firewood imported into WA must be heat-treated to a minimum woodcore temperature of 160o F (71o C) for at least 60 minutes or receive an equivalent WSDA-approved treatment. The wood must also be labeled to show its source & display the statement “Approved Pest Free”. Firewood harvested within Washington State is exempt as are processed wood products, such as compressed wood bricks, wood pellets, logs, or wood products transported for industrial uses, such as to sawmills, pulp & paper mills, & biomass or wood composite facilities. Civil penalties up to $5,000 per violation can be imposed.

The newsletter provides updates on Europe’s double threat: EAB & ash dieback pathogen. 

Europe is home to three species of ash: common ash (Fraxinus excelsior), manna ash (F. ornus), & narrow-leaved ash (F. angustifolia). 

Hungary is the first European Union country with a confirmed EAB infestation (summer 2026). Neighboring Slovakia has also reported EAB presence but this is still unconfirmed.  

While the EAB is native to the Russian Far East & other parts of East Asia, it was not seen west of the Ural Mountains before 2007, when it was reported in western Russia. By 2019 the pest had been recorded in Ukraine & Belarus. Researchers at Ohio State University have found that F. excelsior has at least moderate resistance to EAB.

Fraxinus excelsior in Belgium; photo by Jean-Pol Gramont

The ash decline pathogen (Hymenoscyphus fraxineus) is also from East Asia. It was first described in Poland in 1992 [although probably present much earlier, perhaps the 1990s (Tolio et al., 2025)]. It is now widespread in Europe. Where present, it has killed the vast majority of ash trees. To ascertain whether Oregon ash (Fraxinus latifolia) might be attacked, USDA Forest Geneticist Richard Sniezko of the Dorena Genetic Resource Center has sent seed to European colleagues so that they can plant them and track the results.   

Some good news: British scientists report ~5% of F. excelsior trees appear to exhibit resistance to the parthogen and in some ash groves in northern England ~90% of young seedlings appear to be resistant.

The USDA Forest Service will hold a webinar on Oct. 6th to discuss EAB resistance ash breeding 

Mary Mason, a geneticist w/ USFS Northern Research Station, will present. The webinar starts at 1 PM Eastern Daylight Time on Tuesday, Oct. 6.

Publications named by the Oregon newsletter that are particularly related to the situation in Oregon):

• Hull, C. 2024. A Valley Without Ash: Exploring Strategies for Forested Wetland Restoration Post Emerald Ash Borer Invasion in the Willamette Valley, Oregon. Oregon State University. https://ir.library.ORstate.edu/concern/graduate_projects/3j333b36w

• Melton, A.E., Faske, T.M., Sniezko, R.A., Thibault, T., Williams, W., Parchman, T. & Hamilton, J.A. 2025. Genomics-Driven Monitoring of Fraxinus latifolia (Oregon Ash) to Inform Conservation & emerald ash borer Resistance Breeding. Molecular Ecology e17640. https://doi.org/10.1111/mec.17640  

 • Monitoring Oregon ash forests in the face of the emerald ash borer: A guide for small woodland owners & managers https://extension.ORstate.edu/catalog/pub/em-9451-monitoring-OR-ash-forests-face-emerald-ashborer

• Larval development & parasitism of emerald ash borer (Agrilus planipennis) in Oregon ash (Fraxinus latifolia) & European olive (Olea europaea): implications for the West Coast invasion Journal of Economic Entomology | Oxford Academic

• Maze, D., Bond, J. & Mattsson, M. 2024. Modelling impacts to water quality in salmonid-bearing waterways following the introduction of emerald ash borer in the Pacific Northwest, USA. Biol Invasions (2024). https://doi.org/10.1007/s10530-024-03340-3  

• Kral, G. & D.C. Shaw. 2023. Alternatives to Ash in Western Oregon: With a Critical Tree Under Threat, These Options Can Help Fill Habitat Niche. Oregon State University Extension EM 9396. https://catalog.extension.ORstate.edu/em9396

• Oregon Ash: Insects, Pathogens & Tree Health by Oregon State University Extension (also available in Spanish)  https://extension.ORstate.edu/pub/em-9380  

Useful links for more information

Map to find where EAB is currently confirmed in Oregon: https://experience.arcgis.com/experience/9f29b1860cb04d36ad71b122148277f3

EAB monitoring guidance https://www.OR.gov/odf/forestbenefits/Documents/eab-monitoring-guidance.pdf

Oregon Department of Agriculture https://www.oda.direct/EAB  

Oregon Department of Forestry  https://www.OR.gov/odf/forestbenefits/pages/foresthealth.aspx  

Oregon State University Extension https://extension.ORstate.edu/collection/emerald-ash-borer-resources  

Emerald Ash Borer Information Network, a collaborative effort by the USDA Forest Service & Michigan State University www.emeraldashborer.info  

SOURCE

Tolio, B., P. Sherwood, D. Marčiulynienė, C. Crocoll, M. Cleary, M. Liziniewicz. 2026. Constitutive Metabolite Profiling of European & Asian Fraxinus with Varying Susceptibility to Ash Dieback. Journal of Chemical Ecology 52:8 https://doi.org/10.1007/s10886-025-01678-z

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Wood Packaging: additional information re: continuing introductions

LEAD Technologies Inc. V1.01

Twenty-four years ago the international community adopted ISPM#15 with the aim of reducing forest pest introductions via the wood used to make crates, pallets, and other forms of wood packaging (SWPM). Over that period questions have been raised about its efficacy. See the analyses by Haack et al. I have posted numerous blogs about wood packaging introductions, focused on the United States. To review these, on this website, scroll below the “Archives” to “Categories”, click on “wood packaging”.

Scientists continue to analyze data on wood borer introductions to explore patterns and evaluate the standard’s efficacy. Two recent articles focus on woodwasps in the Siricidae (Nardi et al. 2026) and ambrosia beetles in the Euwallacea complex (Lanschler et al. 2026). Full citations for both are at the end of this blog.

Sirex woodwasps

S. noctilio in Argentina; photo by Paula or Vicki Klasmer via Bugwood

A group of scientist led by D. Nardi surveyed woodwasp introductions to the United States, Canada, and New Zealand to determine historic and current patterns. They found that:

1) Nearly all Sirex woodwasps (84.2% – 97.6%) are transported in wood packaging.

2) While most introductions originated in the woodwasps’ native regions of Europe and Eastern Asia, accompanying high volumes of commodities imported from those regions, interceptions from the Southern Hemisphere have increased recently. Nardi et al. speculate that Asian countries might use softwoods (conifer species) less often for SWPM than do Europe and North America. Certainly the most infamous invasive wood borers from Asia are those that attack hardwoods, e.g., Asian longhorned beetle, emerald ash borer, invasive shothole borers.

3) Widespread adoption of ISPM#15 has significantly reduced interception, establishment, and damage associated with Siricids in the U.S., Canada, and New Zealand since 2002. However, continued detection of live Siricids in wood packaging demonstrates the need for strict enforcement of the standard’s provisions and potentially adoption of additional mitigation strategies.

4) Data collected by phytosanitary agencies of these importing countries is sometimes too limited to support needed analyses of trade patterns and risk. 

  • U.S. phytosanitary agencies identified less than 10% of the intercepted woodwasps to the species level, whereas Canada identified 25% and New Zealand 75%. Identification of the intercepted woodwasp and its country of origin is critical for effective biosecurity. Nardi et al. (2026) express consternation that only 17.8% of interceptions were identified to species level. Even worse, U.S. phytosanitary officials identified less than 10% of the intercepted woodwasps to species. Canadian officials identified 25%, and New Zealand officials identified 75%. Yes, the taxonomy of the family is complex and in flux. And U.S. port staff must process orders of magnitude more interceptions of woodwasps than do either Canada or New Zealand. However, to understand which species are approaching American borders USDA APHIS (which performs the identifications) needs to provide specialized training and apply modern tools e.g., barcoding, molecular diagnostics. CBP and APHIS must also allow adequate time to process the detection before determining the fate of the shipment.
  • U.S. authorities also did not document the country of origin of 83% of shipments associated with Siricid-infested wood packaging intercepted. New Zealand authorities recorded the country of origin of 78% of intercepted shipments, Canadians of 90%.
  • Lack of information on sampling effort impedes exploitation of valuable info. Haack et al. (2014) discuss this obstacle in detail. Nardi et al. (2026) note that changing inspection and reporting priorities – especially when not explicitly described – hamper analysis of which factors explain variations in interception rates over time.

5) Interceptions of Siricids on wood packaging from regions outside the species’ native range have been increasing since the 1960s. Overall, 2.2% of the 504 interceptions named to species level were imported from countries to which they are not native. This included 12.3% of Sirex noctilio (from North America, the Neotropics, and Africa); 3.2% of Urocerus gigas (from North America and the Neotropics). 

These secondary invasions are often from “bridgehead” populations in the Southern Hemisphere. Nardi et al. (2026) worry that such invasion bridgeheads established in trade hubs could speed up biological homogenization of their region.

6) Only a few of the more than 100 species in the family have established in novel regions although many additional species have frequently been intercepted in wood packaging by port inspectors. The species that have established are Sirex noctilio (introduced from Eurasia to North and South America, Australia, New Zealand, and South Africa); and two North American species: Urocerus albicornis (introduced to Europe and Asia) and Sirex obesus to South America. This pattern suggests that biological, environmental, or dispersal barriers interfere with establishment of other Sirex species even when they are transported to new regions.

exotic pine plantation in New Zealand; photo by Jon Sullivan via Flickr
  • One example might be Sirex juvencus. Although it has been intercepted 215 times by one of the three countries, it has not established outside its native range. Nardi et al. (2026) note that the species prefers spruce (Picea spp.), which are much less commonly planted in Southern hemisphere plantations and around the Northen Hemisphere than the pines (Pinus spp.) that support establishment of S. noctilio and U. gigas.
  • The role of the associated fungi is another factor. Nardi et al. (2026) note that another woodwasp species, Xeris spectrum, has not established in New Zealand despite being intercepted often by that country’s phytosanitary officials and presence of suitable hosts. They note that is species does not transport the symbiotic fungi on its body as do other woodwasps. Instead it oviposits on trees already infested with Amylostereum fungus that was injected by an earlier invasive woodwasp.  (A successful biological control program has reduced infestations of S. noctilio, so pine plantations are again widespread on the islands.)

Nardi et al. (2026) warn about several cryptic dangers. First, horizontal transfer of associated symbiont basidiomycete fungal species has been documented: Amylostereum fungal strains from European S. noctilio to American Urocerus species. Such transfers might increase the pathogenicity of formerly benign introductions. Second, scientists don’t yet understand the probable effects of climate change on insect and fungal species’ life cycles. They mention specifically the Asian species Sirex nitobei because its hosts are widespread Pinus species and it has been detected repeatedly, esp. on dunnage.

Nardi et al. (2026) suggest that officials should consider these ecological factors in assessing the risk of new introductions of specific species. I counter that the underlying rationale for adopting ISPM#15 was recognition that trying to manage individual species or countries of origin would not be effective. Instead, I advocate much more assertive enforcement of the standard.

PSHB damage to Harepephyllum caffrum tree in South Africa; photo by Trudy Paap

Invasive shothole borers

Based on analysis on distribution of haplotypes, phylogenetic relationships and dates of first detections, Lantschner et al. (2026) identified seven independent introduction events of the polyphagous shot hole borer (PSHB) Euwallacea fornicatus: to the continental U.S., Hawai`i, South America, Central Europe, Spain, Türkiye, and South Africa. Most apparently originated directly from the species’ native range, although some evidence of likely secondary spread between already invaded regions. Several of these introductions – Israel (2009), South Africa (2016); Brazil (2020), Argentina and Australia (2021), Spain (2022), Uruguay (2023), and Türkiye (2024) – occurred despite stricter biosecurity measures, specifically ISPM#15.

The United States (California) experienced two additional invasions by Euwallaceae in the 2020s: by PSHB E. fornicatus (in San Jose) and a new species, E. interjectus. This makes a total of nine separate introductions.

Lantschner et al. (2026) suggest two opposite explanations for why so many introductions of this group of species from Asia have continued since ISPM#15 came into effect. Their suggestions are that either beetle populations in China, Taiwan, and/or Vietnam grew, thus increasing the pool of potential invaders/propagule pressure, or that increased international exports from these countries opened new commercial pathways. Certainly the latter has occurred. According to Google, exports from China rose from less than $500 billion in 2003 to ~ $4 trillion in 2025. Exports from Vietnam rose from ~$22 billion to $500 billion over the same period.

To be fair, most consider that the principal pathway for movement of species in the Euwallaceae complex is the trade in ornamental plants. In addition to the introductions listed above, E. fornicatus populations have been detected in greenhouses or botanical gardens in Italy, Germany, the Netherlands, and Poland. All have been reported as eradicated (Lantschner et al. 2026). I recently posted a blog discussing the widespread failure of the international phytosanitary system to stem introductions via this trade.

A second group of scientists (Dell, Xu, and Chi 2026) worry that E. fornicatus has spread especially rapidly in South Africa and South America. Already the outbreak of Fusasrium disease in South Africa is the largest the world: it is present in every province except Limpopo. The disease is recorded on 162 tree species, 78 of which are indigenous to the country (Townsend, Hill, Hurley and Roets 2025).

The introduced ranges – sometimes called bridgeheads – create conditions under which the pest can more easily spread further. Lantschner et al. (2026) suggest that the PSHB population established in southern California could spread into the American southeast, eastern Mexico, and parts of Central America. The population in South Africa might expand into other temperate and subtropical regions of Africa. Beetle populations established in Spain, Israel and Türkiye might spread across Mediterranean basin. Population in Western Australia could spread to eastern regions. They note that achieving some of these dispersals would require crossing substantial gaps of unsuitable habitat. They don’t mention that human transport has moved many populations of wood-boring beetles across unsuitable habitat! As I blogged earlier, officials in Sydney, Australia, determined that 47% of trees in the city are vulnerable to PSHB.

SOURCES

Carnegie AJ, Summerell BA, Trollip C, Tovar F, Smith DI and McDonald J (2026) Sentinel trees for early detection of non-native forest pests and pathogens in AU. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Dell, B., W. Xu, and N.M. Chi. 2026. Polyphagous Shot Hole Borer, a Global Threat to Forest Plantations, Green Infrastructure, and Biodiversity: Status, Challenges, and Solutions. Forests 2026, 17, 832

Lantschner, M.V., E. Ceriani-Nakamurakare, A.J. Johnson, A.I. Cognato, S.M. Smith, D.F. Gomez. 2026. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis (Coleoptera: Scolytinae), two global emerging pests. J Pest Sci 99, 100 (2026). https://doi.org/10.1007/s10340-026-02070-w

Nardi, D., K.E. Wagner, S.F. Ward, A.M. Liebhold, E.G. Brockerhoff, R.M. Turner, J.J. Riggins. 2026. Global movement of woodwasps (Hymenoptera: Siricidae) inferred from border interception records Biol Invasions (2026) 28:167 https://doi.org/10.1007/s10530-026-03881-9

Townsend, G., M. Hill, B.P. Hurley, and F. Roets. 2025. Escalating threat: increasing impact of the polyphagous shot hole borer beetle, Euwallacea fornicatus, in nearly all major South African forest types. Biol Invasions (2025) 27:88 https://doi.org/10.1007/s10530-025-03551-2  

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Scientific consensus building: international phytosanitary system is failing, needs to be overhauled

The international movement of plant material, particularly plants for planting, is widely acknowledged as a principal driver of the global eruption of forest health epidemics (Brasier, 2008; Turbelin et al., 2017; Tanney et al. 2025; Burgess and Wingfield 2026). The international plant health (or phytosanitary) community in 2012 adopted ISPM#36, with the goal of reducing pest and pathogen introductions on nursery stock. (“Plants for planting” is the regulatory term for this stock.)  However, the top pages of the International Plant Protection Convention’s (IPPC) website do not mention either this issue or the IPPC’s response – this international standard!

Charles L. Marlatt

Actually, awareness of this risk dates to the 19th Century, at least in Europe. USDA entomologist Charles Marlatt campaigned for the United States to impose phytosanitary rules beginning in 1911. He published a bulletin warning that the U.S. had become a “dumping ground” for contaminated nursery stock from Europe and urged the Congress to act. Marlatt is most famous for requiring destruction of diseased cherry trees sent as a gift by Japan.  Liebhold and Griffin, in their summary of these events,  do not comment on the fact that Marlatt acted without Congressional authority, although destruction of the cherry trees received permission from President Taft. Diplomatic exchanges resulted in Tokyo sending a new batch of pest-free cherries – their descendants grace the Tidal Basin and other parts of Washington, D.C. to this day. At Marlatt’s urging, and following realization of the damage caused by white pine blister rust, Congress adopted the Plant Protection Act in 1912.

This shows that it is possible to protect America’s flora while still enjoying imported plants. But this requires prompt and decisive action, well-prepared in advance, without the likelihood of legal challenges.

Pathogen and Pest Invasions Are Predictable Outcomes

Tanney et al. (2025) say it this way: “We trade not just in plants but also in phytobiomes.” [The phytobiome is the community of microorganisms living on and within a plant.] Burgess and Wingfield (2026) pronounce that invasions are not anomalies but rather predictable outcomes of global commerce interacting with ecological susceptibility. The global nursery trade creates extensive networks that enable the continuous exchange of live plant material across continents. Unlike many others, Burgess and Wingfield (2026) focus not on ornamental horticulture but the repeated occurrence of devastating outbreaks in Eucalyptus and Pinus plantations across the Southern Hemisphere.

Despite a century of efforts to curtail harmful introductions and 70 years after formation of the IPPC, devastating arthropods and disease pathogens continue to be introduced.

Burgess and Wingfield (2026) list the following 11 pathogens introduced since the turn of the 20th Century: Cryphonectria parasitica, Cronartium ribicola, Ophiostoma ulmi/Ophiostoma novo-ulmi and the nematode Bursaphelenchus xylophilus (pine wilt), Phytophthora ramorum, Hymenoscyphus fraxineus, Harringtonia lauricolia, ōhiʻa or myrtle rust (Austropuccinia psidii), and rapid ʻōhiʻa death (Ceratocycstis lukobia and huliohula).

beech leaf disease symptoms, Fairfax County Virginia; photo by F.T.

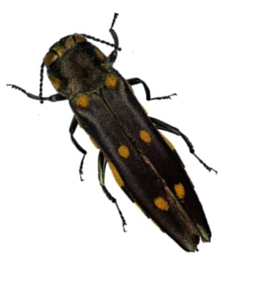
To this list, I add beech leaf disease nematode (Litylenchus crenatae mccannii), the Euwallaceae/Fusarium complex, and, in Europe, lawson cypress root disease, along with numerous arthropods. These include emerald ash borer (Agrilus plannipennis), goldspotted oak borer (Agrilus auroguttatus), Erythrina gall wasp (Quadrastichus erythrinae). All have irreversibly shaped forest ecosystems in their introduced ranges. The forest losses have had numerous repercussions to human societies in the receiving regions.

ohia trees killed by rapid ohia death; photo by Richard Sniezko, USFS

Mitigation Can’t Keep Up Due to System Failures

Tanney et al. 2025 opine that the inevitable conclusion is that past and current mitigation efforts have been insufficient to keep pace. Nor do the failures result only from growing volumes of imports that overwhelm inspection services.

They point to another reason: limited acknowledgment and integration of phytobiome-associated risks into regulatory frameworks. The system ignores particularly fungal endophytes and latent pathogens with extended asymptomatic or presymptomatic phases.

Their telling illustration is the ash decline epidemic in Europe. Hymenoscyphus fraxineus is a harmless endophyte–saprotroph on its native Asian host (Fraxinus mandshurica). However, it was introduced to the naïve host European ash (Fraxinus excelsior), on which it became an aggressive necrotrophic pathogen that has killed millions of trees. Even if the organism had been detected (the authors thought this unlikely) before the outbreak was recognized, the detection would not have triggered a risk assessment or any phytosanitary measures. None of the approximately 200 species in the genus had been reported as a pathogen. In fact, a congener, H. albidus, has a similar endophyte– saprotroph life cycle on European ash without causing harm.

McTaggart et al. (2016) flagged these issues a decade ago. They said that recent advances in gene sequencing technologies reveal a vast diversity of fungi causing asymptomatic infections. Some are endophytes, defined as fungi that, for all or part of their life history, asymptomatically colonize plant tissue. Some are pathogens with extended asymptomatic stages. When introduced to naïve hosts, some of either can erupt. Therefore, international phytosanitary measures, including the one significant effort to address the plants for planting pathway, ISPM#36, should focus more on phytobiomes as a biosecurity concern. (See my blog reporting Dr. Eliana Torres Bedoya on this topic.)

Tanney et al. (2025) are not alone in calling out the system’s failure. See Weed, Ayres, and Hicke (2013), Fei et al. (2019), Quirion et al. (2021) for North America; and Gougherty, Sitzia et al. (2021) and Martinac et al. (2025) for a global perspective. Raffa et al. (2023) say national and international phytosanitary policies and programs must reflect the true level of threat from introduced plant pathogens (of all Phyla and Kingdoms) and scientific limits.

Experts on ambrosia beetles – insects that have symbiotic relationships with fungi – say the same. Dell, Xu and Chi 2026 call for studies of Euwallaceae fornicatus’s broader phytobiome, especially bacterial communities, which are increasingly recognized as important components of the ambrosia beetle system.

Nor are Tanney et al. (2025) alone in calling on phytosanitary officials to stop using methods known to fail. That is, relying on visual inspections of plants and basing decisions on whether a pest has previously been designated.

A decade ago McTaggart et al. (2016) called for shifting from a name-based to a gene-based biosecurity risk mitigation approach. Burgess and Wingfield (2026) say officials must move beyond case-by-case responses to embrace broader preventative approaches that address the underlying mechanisms of pathogen emergence and spread.

As Tanney et al. (2025) and Bonello describe, the current international phytosanitary framework relies on symptomatic hosts carrying named pathogens. This approach ignores the facts:

  1. endophytes and latent pathogens with prolonged asymptomatic phases are
    1. ubiquitous – on and in leaves, buds, inflorescences, fruit, seeds, xylem, phloem, cambium, and bark. Phytobiomes are more species-rich on plants lacking disease symptoms.
    1. diverse – fungi, bacteria, viruses, nematodes. Some are known pathogens.
    1. challenging to identify. They often can’t be isolated using standard lab processes. If the genome has not already been sequenced and recorded in databases even sequencing-informative loci or barcodes might fail to identify the taxa. (Only ~150,000 species of an estimated 2.5 million fungi are so compiled.)
    1. in some cases, a significant threat to forest health when introduced to naïve realms.
  2. Scientists cannot predict impacts that might accompany introduction of nearly any of these organisms to a naïve host. Missing information pertains, inter alia, to endophyte identities and life histories, trees’ defenses, and the effects of the current and changing climate.
  3. Host ranges might shift during an organism’s life cycle, e.g., juvenile vs. mature/reproducing.
  4. Host jumps within the same host genus are likely (Tanney et al. 2025). They say that importing living plant into areas with congeneric endemic plants is highly risky.
  5. Most endophytes in woody plants can be horizontally transmitted by abiotic (e.g., wind, rain, and surface water movement) transmission and biotic (e.g., insect) vectors. Every colonized leaf might be a propagule! (Tanney et al. 2025)
  6. Microbes might reproduce both asexually and sexually. Sometimes dispersal of these propagule uses different modes, e.g., insect- and water-dispersed asexual spores combined vs. air-dispersed sexual spores.
  7. Endophytes can switch from being asymptomatic to pathogenic when hosts are stressed. Tanney et al. (2025) name several examples, including Fusarium circinatum – causal agent of pine pitch canker.

To protect our plant resources – in forests, in agricultural fields, in our gardens – scientists must be empowered to develop methods and policies that better account for unnamed and unknown organisms.

Tanney et al. (2025) note that there is some flexibility in the face of unknown threats. The World Trade Organization’s Agreement on the Application of Sanitary and Phytosanitary Standards (SPS Agreement) and ISPM#2 allow adoption of a temporary phytosanitary measure based on the information available, even when it is limited. APHIS’ NAPPRA program link takes this approach. I think countries could use this flexibility more often. (I discuss the SPS and IPPC system in greater detail in my report Fading Forests II. I provide a link at the end of this blog.)

How to Improve Prevention

Some progress has been made in countering introductions of arthropods. Adoption of ISPM#15 regulates an entire pathway (crates, pallets, and other forms of packaging made from wood). CISP applauds the approach but calls for more aggressive enforcement. (On this website, scroll down below “Archives” to “Categories”, click on “wood packaging”). I note that introductions via this pathway nevertheless continue: Lantschner et al. (2026) have identified seven independent introductions of Euwallacea fornicatus. Introductions to San Jose, California; Israel; South Africa; Brazil; Spain; and Türkiye occurred after most countries had begun implementing ISPM#15. The same is true of the introduction of the congener E. kuroshio to southern California. Nardi et al. (2026) demonstrate continuing introductions of woodwasps in wood packaging.

Unlike wood products, imported plants, especially those intended to be planted in the new location, must remain alive and healthy. It is extremely challenging to devise effective treatments to kill the arthropod or pathogen without harming the plant. Tanney et al. (2025) discuss the pros and cons of several options, including ionizing radiation, fungicide treatments, and various heat treatments. They note that more research is needed to assess the feasibility, efficacy, optimal dosage, and potential risks of devitalizing plants in high-throughput treatments.

New Tools for Prevention

So the focus remains on preventing introductions. Fortunately, new tools make possible new approaches.

Detection of Pathogens — Tanney et al. (2025), Carnegie et al. (2026), Burgess and Wingfield 2026, and Bonello (pers. comm.) point to the suite of new molecular, remote sensing, and artificial intelligence tools becoming usable for detecting pathogens. They and Dell, Xu and Chi (2026) stress that citizen science can extend the reach of formal surveillance.

Rapid Responses — Tanney et al. (2025) and Carnegie et al. (2026) concede that more work is needed to address such considerations as detecting DNA from nonviable cells, and to develop international standards. However, they assert that results from these tools are already sufficiently science-based to inform decision-making, specifically to implement rapid responses including precautionary quarantines and other measures along with intensive surveys and conducting triage assessments.

Inspection and Enforcement — Burgess and Wingfield (2026) call more generally for enforcing comprehensive phytosanitary treatments and certifications for the live plant and timber trades, and focusing inspection efforts on high-risk entry points. Port detection can be sped up and improved by applying rapid molecular diagnostic tools.

Risk Assessments — New tools and approaches can also improve risk assessments. I blogged earlier about advances in predicting which trees are likely highly damaged, if certain pest insects are introduced. See Mech et al. 2019; Raffa et al. 2023; Schulz et al. 2025; Uden et al. 2022. This is encouraging, although additional work on arthropods is still needed. Carnegie et al. (2026) and Hulcr (2026, USDA Interagency Symposium on Invasive Species, Annapolis Maryland) both note the need for continued investment in taxonomic surveys to generate baseline data.

Predicting the probable impacts of introduced pathogens is inherently more difficult.

  • After introduction to novel systems pathogens sometimes evolve rapidly and becoming more aggressive and difficult to manage (Burgess and Wingfield 2026).
  • Host jumps within the host genus are likely. This exacerbates the risk arising from importing living plants into areas with congeneric endemic plants. Under these circumstances the risk assessment must be especially careful in balancing economic and social benefits of trade w/ potential ecological, economic, and social consequences of invasion (Tanney et al. 2025; Burgess and Wingfield 2026). Tanney et al. (2025) recommend systematic studies of regularly traded species from areas of origin (or sites of production) to eventual destinations to provide a foundation for assessing the risk of phytobiomes arriving on imported plants. These studies would also help to determine effectiveness of management approaches.

A number of authors are exploring how to address these difficulties. For example, Tanney et al. (2025) advise using “omics”-based approaches to predict invasiveness, virulence, and host interactions. Caveat: same genes are present regardless of whether the organism is an endophyte on its native host or a pathogen on a naïve host. At the same time, host response must be assessed by combining omics-based approaches, sentinel plantings, and modeling.

Tanney et al. (2025) also recommend greatly expanding sentinel planting-based surveillance.  Sentinel plant systems must be carefully managed to provide the necessary levels of information. Raffa et al. (2023) nivemdiscuss strengths and weaknesses of this approach. Eliana Torres Bedoya and Enrico Bonello blog warn that sentinel plantings must support screening all plant parts, above and below-ground, for all potentially pathogenic taxa, including nematodes, phytoplasmas, and viruses. Furthermore, samples must be analyzed from asymptomatic plants, not just those showing signs of disease. Finally, samples must be collected throughout the year. Carnegie et al. (2026) call for greater coordination within the country and with international colleagues (e.g., through the International Plant Sentinel Network (IPSN).

Tanney et al. (2025) provide a convenient list of approaches they think will help close the knowledge gaps that challenge integrating attention to phytobiomes into phytosanitary decision-making.  

Tanney et al. (2025) and Burgess and Wingfield (2026) advocate shifting the focus of risk assessments from specific pests to commodity-based or pathway risk assessments that consider unknown but plausible threats.

Horizon scanning is often described as helpful in predicting the next invasion. However, I have been disappointed by the usefulness demonstrated by some applications of the approach – at least in the absence of policies and resources to support a robust “rapid response”. At least in Cyprus blog and the United Kingdom, the main response to detection of one of the predicted species is only heightened monitoring — not attempted management!! According to Peyton et al. (2026), the British exercise failed to evaluate 78% of the 112 species that were introduced over the following decade. The vast majority were not evaluated because they were expected to have negligible impacts on biodiversity in Britain — but some turned out to be damaging.

Countries also need current data on which to base analyses and determine efficacy of programs. I regret that all American analyses of the risk associated with imported “plants for planting” rely on data collected by Liebhold et al. (2012) — which is from 2009!! Not only are these data 17 years old; APHIS has made major changes to its regulations in the interval — including implementation of the NAPPRA program.

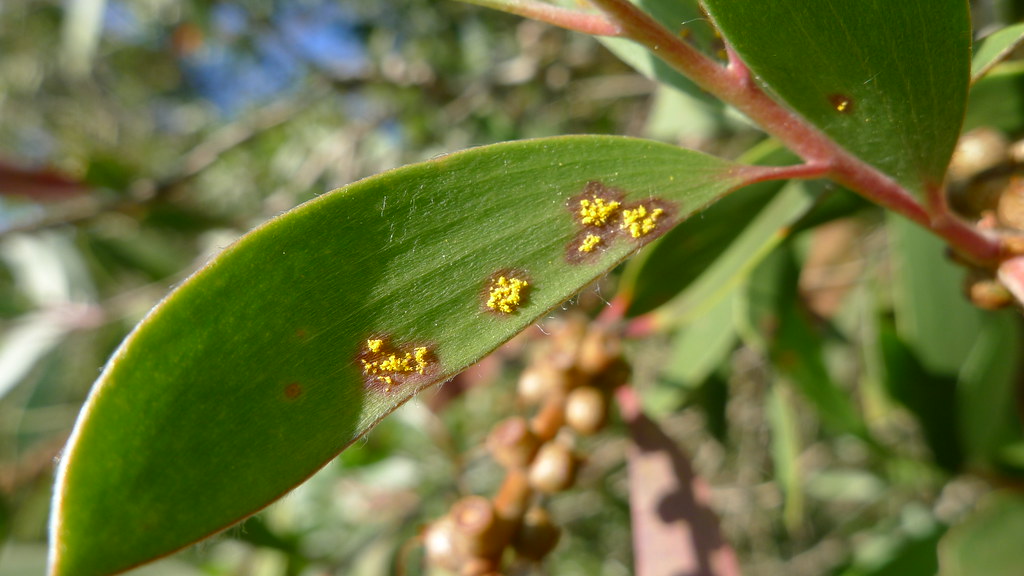
The missing component often is rapid response – often justified by uncertainty regarding the introduced organism’s possible impacts.Wingfield and Burgess (2026) cite the example of Australia’s weak response to detection of myrtle rust, Austropuccinia psidii. Now established in the rainforests of eastern Australia (states of New South Wales, Queensland, and Victoria) and an outbreak in Western Australia, myrtle rust threatens at least 76 species. Australia is home to 38% of all species in the vulnerable Myrtaceae family (Carnegie et al. 2026).

myrtle rust on Melaleuca tree in Australia; photo by John Tann via Flickr

Burgess and Wingfield (2026) cite several lessons based on the Northern Hemisphere’s experience with pathogen introductions. They call specifically for more stringent phytosanitary standards, advanced diagnostic techniques, and risk-optimized surveillance. These should be backed up by collaborative resistance breeding programs for high-risk hosts. They note the need for international cooperation across science, policy, industry, and communities.

Proposed Amendments to Trade Regulations

Tanney et al. (2025) point to the value of shifting to a system that favors trading in propagative material with subsequent bulking up in the importing countries for domestic consumption. (See also my advocacy in Fading Forests II.) They concede that this approach is unlikely to be implemented. As a fallback, they suggest applying this approach to the highest-risk commodities, e.g., rhododendron plants. They note that these plants have transported Phytophthora ramorum.

Scientific Fields

Burgess and Wingfield (2026) point to the need for multidisciplinary research to integrate forest pathology with chemical, ecological and social sciences to anticipate pest emergence. I add: integrating plant pathology with invasion science. The two disciplines rarely interact. Paap et al. (2020) suggest a framework to bridge this gap. I noted that the recent IUCN survey regarding the need for an updated species conservation strategy, while it incorporates invasive species issues, did not mention regional phytosanitary organizations, such as EPPO or NAPPO, among the bodies with whom invasions scientists should build relationships.

Interestingly, a group of experts on invasive plants (Hulme et al. 2026) are trying to expand relationships among researchers even more broadly. They seek to integrate invasion science into on-going discussion of global megatrends. Megatrends are clusters of interdependent global trends observed today that together have the potential to cause significant shifts in environmental, economic, and social conditions. At present, government, industrial, and other leaders evaluating how societies might adapt to these changes are not even considering their probable effect on bioinvasions. At least bioinvasion scientists are starting to evaluate the effects of the megatrends.

The invasion scientists explored how 15 megatrends might affect arrival, establishment, spread, and impacts (environmental and economic) of invading non-native plants over the next 25 years. They grouped the trends into four larger gigatrends: “Anthropocene”, “Digital”, “Societal”, and “Technology”.

They expect most of the megatrends to increase invasion risks, especially by accelerating species arrival and spread. While trends grouped under “Technology” promise some improvements in detection and control tools, there are significant barriers to their adoption. This worrying statement should be addressed by the proponents of applying these measures I cited earlier.

Hulme et al. (2026) urge invasion scientists to persuade policymakers that by taking decisive action to steer these trajectories toward mitigating the growing global threat of bioinvasion.

The Need for Adequate Funding and Political Support

Burgess and Wingfield (2026) note that risk assessment, inspection, detection, and response programs need to be supported by investment in quarantine infrastructure, diagnostic laboratories, and emergency response funds to enhance readiness for new incursions.

As they stress, prevention and preparedness cannot rest solely with scientists. Political commitment, regulatory authority, and industry engagement are indispensable. The efforts need the active participation of affected economic sectors, and sustained investment by governments, scientific institutions,  industry, and society. The need for reliable, long-term funding and societal support is shared with all invasive species programs. Nearly all participants in the IUCN survey ranked this need at the top.

Property owners, the wood products and nursery industries, and governments from municipal to national have incurred substantial economic costs. Entire wooded ecosystems have been destroyed. Affected stakeholders, however, have not demanded that officials adopt more effective plant health  strategies to reduce this risk. Scott Schlarbaum and I have released three “Fading Forest” reports trying to make this happen (links provided below). As shown here, many scientists are calling for action. To quote the late Congressman John Lewis in the context of civil rights, “If not now, when? If not you, who?”

SOURCES

Burgess, T.I. and M.J. Wingfield. 2026. Unveiling a Hidden Menace: Invasive Tree Pathogens, Less Known but Increasingly Threatening Southern Hemisphere Forests Annual Review of Phytopathology 64:18.1–18.2664:18.1–18.26

Carnegie, A.J., B.A. Summerell, C. Trollip F. Tovar, D.I. Smith, and J. McDonald.  2026. Sentinel trees for early detection of non-native forest pests and pathogens in Australia. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Dell, B., W. Xu, and N.M. Chi. 2026. Polyphagous Shot Hole Borer, a Global Threat to Forest Plantations, Green Infrastructure, and Biodiversity: Status, Challenges, and Solutions. Forests, 17, 832

Fei, S., R.S. Morin, C.M. Oswalt, & A.M. 2019. Biomass losses resulting from insect & disease invasions in United States forests

Gougherty, A.V. & Davis,T.J. (2024) Evolutionary history of host trees amplifies the dilution effect of biodiversity on forest pests.  PLoSBio. 22(2):e30024730 https://doi.org/10.1371/journal.pbio.3002475 PLOSBiology |https://doi.org/10.1371/journal.pbio.3002473 February 27, 2024 1 / 1

Hulme, P.E., J.N. Barney, J.L. Bufford, J.A. Catford, J.A. Coetzee, C.C. Daehler, M.S. Dechoum, H. Jäger, A.  Pauchard, P. Pyšek, D.M. Richardson, M. Vilà, E. Wandrag, J.R.U. Wilson. 2026. Seeds of change: Global megatrends will shape the future trajectory of plant invasions. BioScience , 2026, https://doi.org/10.1093/biosci/biag096

Lantschner, M.V., E. Ceriani-Nakamurakare, A.J. Johnson, A.I. Cognato, S.M. Smith, D.F. Gomez. 2026. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis (Coleoptera: Scolytinae), two global emerging pests. J Pest Sci 99, 100 2026. https://doi.org/10.1007/s10340-026-02070-w

Liebhold, A.M., E.G. Brockerhoff, L.J. Garrett, J.L. Parke, and K.O. Britton. 2012. Live Plant Imports: the Major Pathway for Forest Insect and Pathogen Invasions of the US. www.frontiersinecology.org

Martinac, M-L., F. Ningre, A. Dowkiw, N.Le Goff, B. Marcais. 2025.  High host density favour ash dieback. Plant Pathology 2025, 74 (5)  10.1111/ppa.14099

Martinou, A.F., J. Demetirou, I. Angelidou, N. Kassinis, A. Melifronidou, J.M. Peyton, H.E. Roy, A.N.G. Kirschel. 2026. Multiple introductions of invasive alien species on a Mediterranean island predicted by horizon scanning. Biological Invasions 2026 28:41 https://doi.org/10.1007/s10530-025-03729-8

McTaggart, A.R., M.A. van der Nest, E.T. Steenkamp, J. Roux, B. Slippers, L.S. Shuey, et al. (2016) Fungal Genomics Challenges the Dogma of Name-Based Biosecurity. PLoS Pathog 12(5): e1005475. doi:10.1371/journal.ppat.1005475

Mech,  A.M., K.A. Thomas, T.D. Marsico, D.A. Herms, C.R. Allen, M.P. Ayres, K.J. K. Gandhi, J. Gurevitch, N.P. Havill, R.A. Hufbauer, A.M. Liebhold, K.F. Raffa, A.N. Schulz, D.R. Uden, & P.C. Tobin. 2019. Evolutionary history predicts high-impact invasions by herbivorous insects. Ecology & Evolution 9(21): 12216–12230. https://doi.org/10.1002/ece3.5709

Nardi, D., K.E. Wagner, S.F. Ward, A.M. Liebhold, E.G. Brockerhoff, R.M. Turner, J.J. Riggins. 2026. Global movement of woodwasps (Hymenoptera: Siricidae) inferred from border interception records Biol Invasions (2026) 28:167 https://doi.org/10.1007/s10530-026-03881-9

Paap, T., M.J. Wingfield, T.I. Burgess, J.R.U. Wilson, D.M. Richardson, and A. Santini. 202 Harmonising the fields of invasion science and forest pathology NeoBiota Vol 62 2020 pages 301-332

Peyton, J.M., S. Rorke, D.C. Aldridge, O.L. Pescott, K. Dehnen- Schmutz, D.G. Noble,  J. Sewell, A.J.A. Stewart,  T. Adriaens,  B.C. Beckmann,  J. R. Britton, J. Brodie1, P.M.J. Brown, I.C.N. Cavadino, P.F. Clark, A.M. Dunn, J.Foster, C. Harrower, M.C. Harvey, M.C. Jackson, T. Jones, C.A. Maggs, G. Martin, F. Mathews, A.C. Mill, D. Murphy,  E. Paganini, R. Payne, W. Rabitsch, T. Renals,    K. Schönrogge, R.H. Shaw, G.C. Smith, P.D. Stebbing, P.A. Stroh, H. Tidbury, E. Tricarico, J. Vallet,   K.J. Walker, L.E. Wood, C.A. Wood, B. Woodcock, H.E. Roy. 2026. Assessing the success of a horizon scanning approach in predicting invasive non-native species arrival. J Appl Ecol. 2026; 63: https://doi.org/10.1111/1365-2664.70217

Quirion BR, Domke GM, Walters BF, Lovett GM, Fargione JE, Greenwood L, Serbesoff-King K, Randall JM & Fei S (2021) P&P Disturbances Correlate With Reduced Carbon Sequestration in Forests of the Contiguous US. Front. For. Glob. Change 4:716582.  [Volume 4 | Article 716582] doi: 10.3389/ffgc.2021.716582

Rabaglia, R.J., S.A. Dole, and A.I. Cognato. 2006. Review of American Xyleborina (Coleoptera: Curculionidae: Scolytinae) Occurring North of Mexico, with an Illustrated Key. Ann. Entomol. Soc. Am. 99: 1034–1056.

Raffa, K.F., E.G. Brockerhoff, J-C. Gregoirem, R.C. Hamelin, A.M. Liebhold, A. Santini, R.C. Venette, and M.J. Wingfield. 2023. Approaches to Forecasting Damage by Invasive Forest Insects and Pathogens: A Cross-Assessment. Bioscience Vol. 73, No. 2. February 2023.

Schulz, A.N., N.P. Havill, T.D. Marsico, M.P. Ayres, K.J.K. Gandhi, D.A. Herms, A.M. Hoover, R.A. Hufbauer, A.M. Liebhold, K.F. Raffa, K.A. Thomas, P.C. Tobin, D.R. Uden, A.M. Mech. 2025. What Is a Specialist? Quantifying Host Breadth Enables Impact Prediction for Invasive Herbivores Ecology Letters 28: e70083. https://doi.org/10.1111/ele.70083

Tanney, J.B., M. Kemler, M. Vivas, M.J. Wingfield, and B. Slippers. 2025. Silent invaders: the hidden threat of asymptomatic phytobiomes to forest security. New Phytologist 2025 247: 533–545 doi: 10.1111/nph.70209

Uden, D.R., A.M. Mech, N.P. Havill, A.N. Schulz, M.P. Ayres, D.A. Herms, A.M. Hoover, K.J.K. Gandhi, R.A. Hufbauer, A.M. Liebhold, T.D. Marsico, K.F. Raffa, K.A. Thomas, P.C. Tobin, C.R. Allen. 2022. Phylogenetic risk assessment is robust for forecasting the impact of European insects on No Am conifers. Ecological Applications 33(2): e2761. https://doi.org/10.1002/eap.2761

Weed, A.S., M.P. Ayers, J.A. Hicke. 2013. Consequences of climate change for biotic disturbances in North American forests. Ecological Monographs, 83(4), 2013, pp. 441–470

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

New Zealand kauri – essential to mitigating climate change

a large kauri tree on New Zealand’s North Island; photo by F.T. Campbell

I applaud the growing attention to the impacts of deadly pathogens in forests. The focus is often on the resulting decrease in tree-based storage of atmospheric CO2. In an earlier blog I cited findings by Quirion et al. (2021) that forest diseases in the United States between 2001 and 2019 reduced mean forest carbon sequestration by 28%. Forests were converted from carbon storage to carbon sources. [Full citations for all sources provided at the end of this blog.] Earlier, Fei et al. (2019) had determined that compensatory growth by non-host species (spurred by reduced competition and greater resource availability after a dominant tree species dies) might partially offset CO2 decline, although only over long timescales.  Chan et al. (2026) cite examples from redwoods in California to Dipterocarps in Southest Asia that document the importance of large trees in sequestering atmospheric CO2. See also Calders et al. re: Wytham Woods in the United Kingdom.

A pertinent current example is found in New Zealand. There, the oomycete Phytophthora agathidicida is killing the endemic kauri tree, Agathis australis. Kauri are among the largest and longest-lived trees on Earth. The average age of large individuals in old-growth stands is ~ 600 years; exceptional specimens reach 1,600 years. Typical diameters in old-growth stands are 1.3–1.5 m; exceptional specimens > 7 meters (Chan et al. 2026).

A year ago Simpkins et al. (2025) reported a modeling study that indicated that kauri dieback disease could cause a decrease in aboveground carbon stocks by 55% over 500 years. However, as Chan et al. (2026) point out, stand-level carbon sequestration and storage in a forest undergoing widespread mortality of the dominant tree species depend on growth and productivity of the replacement species. Even the magnitude of short-term dynamics depends on the relative abundance of the vulnerable host and the rate of its mortality and decline.

Therefore they explored the impact of kauri dieback in greater detail, including which species they thought likely to replace kauri and their carbon-sequestration capabilities at the stand level.

Although (regrettably) not the focus of their article, Chan et al. (2026) note that loss of the kauri tree also threatens biodiversity. Kauri strongly modify their environment through accumulation of a thick organic soil layer derived from litter. The layer is typically 30 to 50 centimeters deep but can reach 2 meters. These soils are acidic, drought-prone and nutrient-poor. As result the co-occurring plants comprise a unique suite of stress-tolerant plants. The vertical stratification of conifer and angiosperm crowns in kauri forests allows coexistence and unusually high total basal area of other plant species.

In these forests, kauri have dominated annual CO2 capture and long-term storage. Under pre-invasion conditions, Chan et al. (2026) this to continue. Previous work estimated that live vegetation biomass in kauri stands doubles when the stand moves from early- or mid-successional stages to mature. Three other species each contribute more than 10% of carbon storage: the tree fern Cyathea dealbata, and two small trees, Phyllocladus trichomanoides and Kunzea ericoides. All are early successional species that typically dominate in open or disturbed environments but decline as canopies close.

Chan et al. (2026) studied changes in live vegetation carbon stocks between two census periods ten years apart, 2011 – 2014 and 2021 – 2024. The five kauri-dominated plots included two plots each in early- and late-successional stages and one mid-successional stand. The study site was in the greater Auckland region of North Island. Phytophthora agathidicida is spreading through these forests, infecting kauri of all ages. Still, dieback intensity varies within the plots, so they were subdivided plots into 20 10 m × 10 m subplots.

Chan et al. (2026) tried to measure two distinct processes: the increase in carbon stocks coming from recruitment and growth of live stems (= productivity) and loss of sequestration and storage due to tree mortality. The two phenomena might respond differently to kauri dieback and initial carbon stocks. While increasing disease severity and increased mortality both result in lower net accumulation, it is important to disentangle the effects of increased loss, reduced productivity, or the combination.

kauri killed by dieback disease; 149 kauri dieback 02-868×1300

Findings

Carbon sequestration declined proportionately with increasing disease severity due to both reduced productivity and greater carbon loss from mortality. Because kauri contributed the largest share of carbon sequestration and storage due to the enormous size of some individuals, death of higher numbers of large kauri led to the largest reductions in these services. That is, the greatest observed decrease in carbon sequestration and storage was in those stands that initially had the highest levels of carbon storage. These were stands in mid- and late-successional subplots rather than in early-successional subplots. The higher the initial mean carbon stock level, the more pronounced the observed decline in sequestration.

This means that kauri dieback threatens both the carbon sequestration and long-term carbon storage capacity of kauri forests, particularly in mature stands comprising the largest trees.

Chan et al. (2026) conclude that the carbon stocks of these mature kauri stands will not stabilize until after substantial depletion of kauri biomass. As a result, long-term carbon storage capacity is markedly reduced.

Meanwhile, healthy kauri stands continued to sequester carbon as the trees grew. Chan et al. (2026) expect living kauri trees to continue adding to their basal area and other productive species can co-exist under the vertically stratified crowns.

In stands that had low carbon sequestration levels at the time of the first census (early successional stands), the stand maintained positive carbon sequestration until the disease reached a higher intensity. This was because some of the other tree species in the stand raised their proportional contributions to CO2 sequestration. Chan et al. (2026) concluded that these stands were likely stabilize at a reduced level of biomass, effectively lowering their long-term carbon storage and sequestration potential.

The steep decline in carbon sequestration and storage associated with higher initial carbon stocks reveal the disproportionate vulnerability of mature kauri stands. The kauri contribution to stand biomass is unlikely to be replaced by a structurally similar species, e.g., the long-lived, large conifer rimu (Dacrydium cupressinum), until passage of many years. Early-successional species are expected to colonize the damaged forests rapidly, but their lower wood densities and fast maturity/senescence confer limited carbon storage capacity.

a rimu tree; photo by F.T. Campbell

Besides, some of the species likely to replace (temporarily) dead kauri — Myrtaceae such as Kunzea ericoides — are susceptible to another introduced pathogen, myrtle rust (Austropuccinia psidii) (Lantham et al. 2025).

So kauri dieback not only reduces current carbon stocks but succession dynamics do not support future sequestration potential, leading to a long-term decline in the carbon storage capacity of these forests. 

Chan et al. (2026) call for urgent efforts to prevent spread of the pathogen Phytophthora agathidicida and injection of phosphite to reduce disease symptoms. Both strategies should target mature kauri stands. Research on phosphite treatments is under way. They also suggest research on disease progression and associated changes in carbon stocks across multiple pools, including coarse and fine woody debris and deep organic soil layers.

Chan et al. (2026) report that the disproportionate contribution of large, long-lived individual trees to carbon storage is a worldwide phenomenon.

Extraneous thought: I am glad that Chan et al. (2026) cite examples of high-impact pathogens from the Southern Hemisphere, i.e., Phytophthora cinnamomi in Australia. While chestnut blight certainly had severe impacts, so have many others, e.g., white pine blister rust Cronartium ribicola. Some arthropods have also proved damaging on several continents, including emerald ash borer (Agrilus plannipennis), or across widely separated island systems, e.g., Erythrina gall wasp (Quadrastichus erythrinae) and cycad scale (Aulacaspis yasumatsui). I regret that I can find no recent information on the scale.

SOURCES

Calders, K., H. Verbeeck, A. Burt, N. Origo, J. Nightingale, Y. Malhi, P. Wilkes, P. Raumonen, R.G.H. Bunce, M. Disney.  Laser scanning reveals potential underestimation of biomass carbon in temperate forest. Ecol Solut Evid. 2022;3:e12197. wileyonlinelibrary.com/journal/eso3

Chan, P.J., T. Elliott, H.R. Lai, B. Burns, L. Schwendenmann. 2026. Consequences of a dieback disease on carbon stocks and fluxes in forests dominated by a susceptible foundation species. Plant Ecology  (2026) 227:97 https://doi.org/10.1007/s11258-026-1669-4

Fei, S, R.S. Morin, C.M. Oswalt, and A.M. Liebhold. 2019. Biomass losses resulting from insect and disease invasions in US forests. Proceedings of the National Academy of Sciences. August 27, 2019 vol. 116  no. 35 www.pnas.org/cgi/doi/10.1073/pnas.1820601116

Latham, M.C., A. Lustig, N.M. Williams, A. McDonald, T. Patuawa, J. Chetham, S. Johnson, A. Carrington, W. Wood, and D.P. Anderson. 2025.  Design of risk-based surveillance to demonstrate absence of Phytophthora agathidicida in NZ kauri forests. Biol. Invasions (2025) 27, no.26 https://doi.org/10.1007/s10530-024-03501-4

Quirion BR, Domke GM, Walters BF, Lovett GM, Fargione JE, Greenwood L, Serbesoff-King K, Randall JM and Fei S (2021) P&P Disturbances Correlate With Reduced Carbon Sequestration in Forests of the Contiguous US. Front. For. Glob. Change 4:716582.  [Volume 4 Article 716582 doi: 10.3389/ffgc.2021.716582

Simpkins, C.E., P.J. Bellingham, K. Reihana, J.M.R. Brock, G.L.W. Perry. 2024. Evaluating the effects of two newly emerging plant pathogens on North Aotearoa-NZ forests using an individual-based model.  Ecological Modelling, www.elsevier.com/locate/ecolmodel https://doi.org/10.1016/j.ecolmodel.2024.110938

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

See also my earlier blog about the vulnerability of the seven unique floral kingdoms of the Southern Hemisphere  

Southern Hemisphere forests: unique biomes face high invasion risk

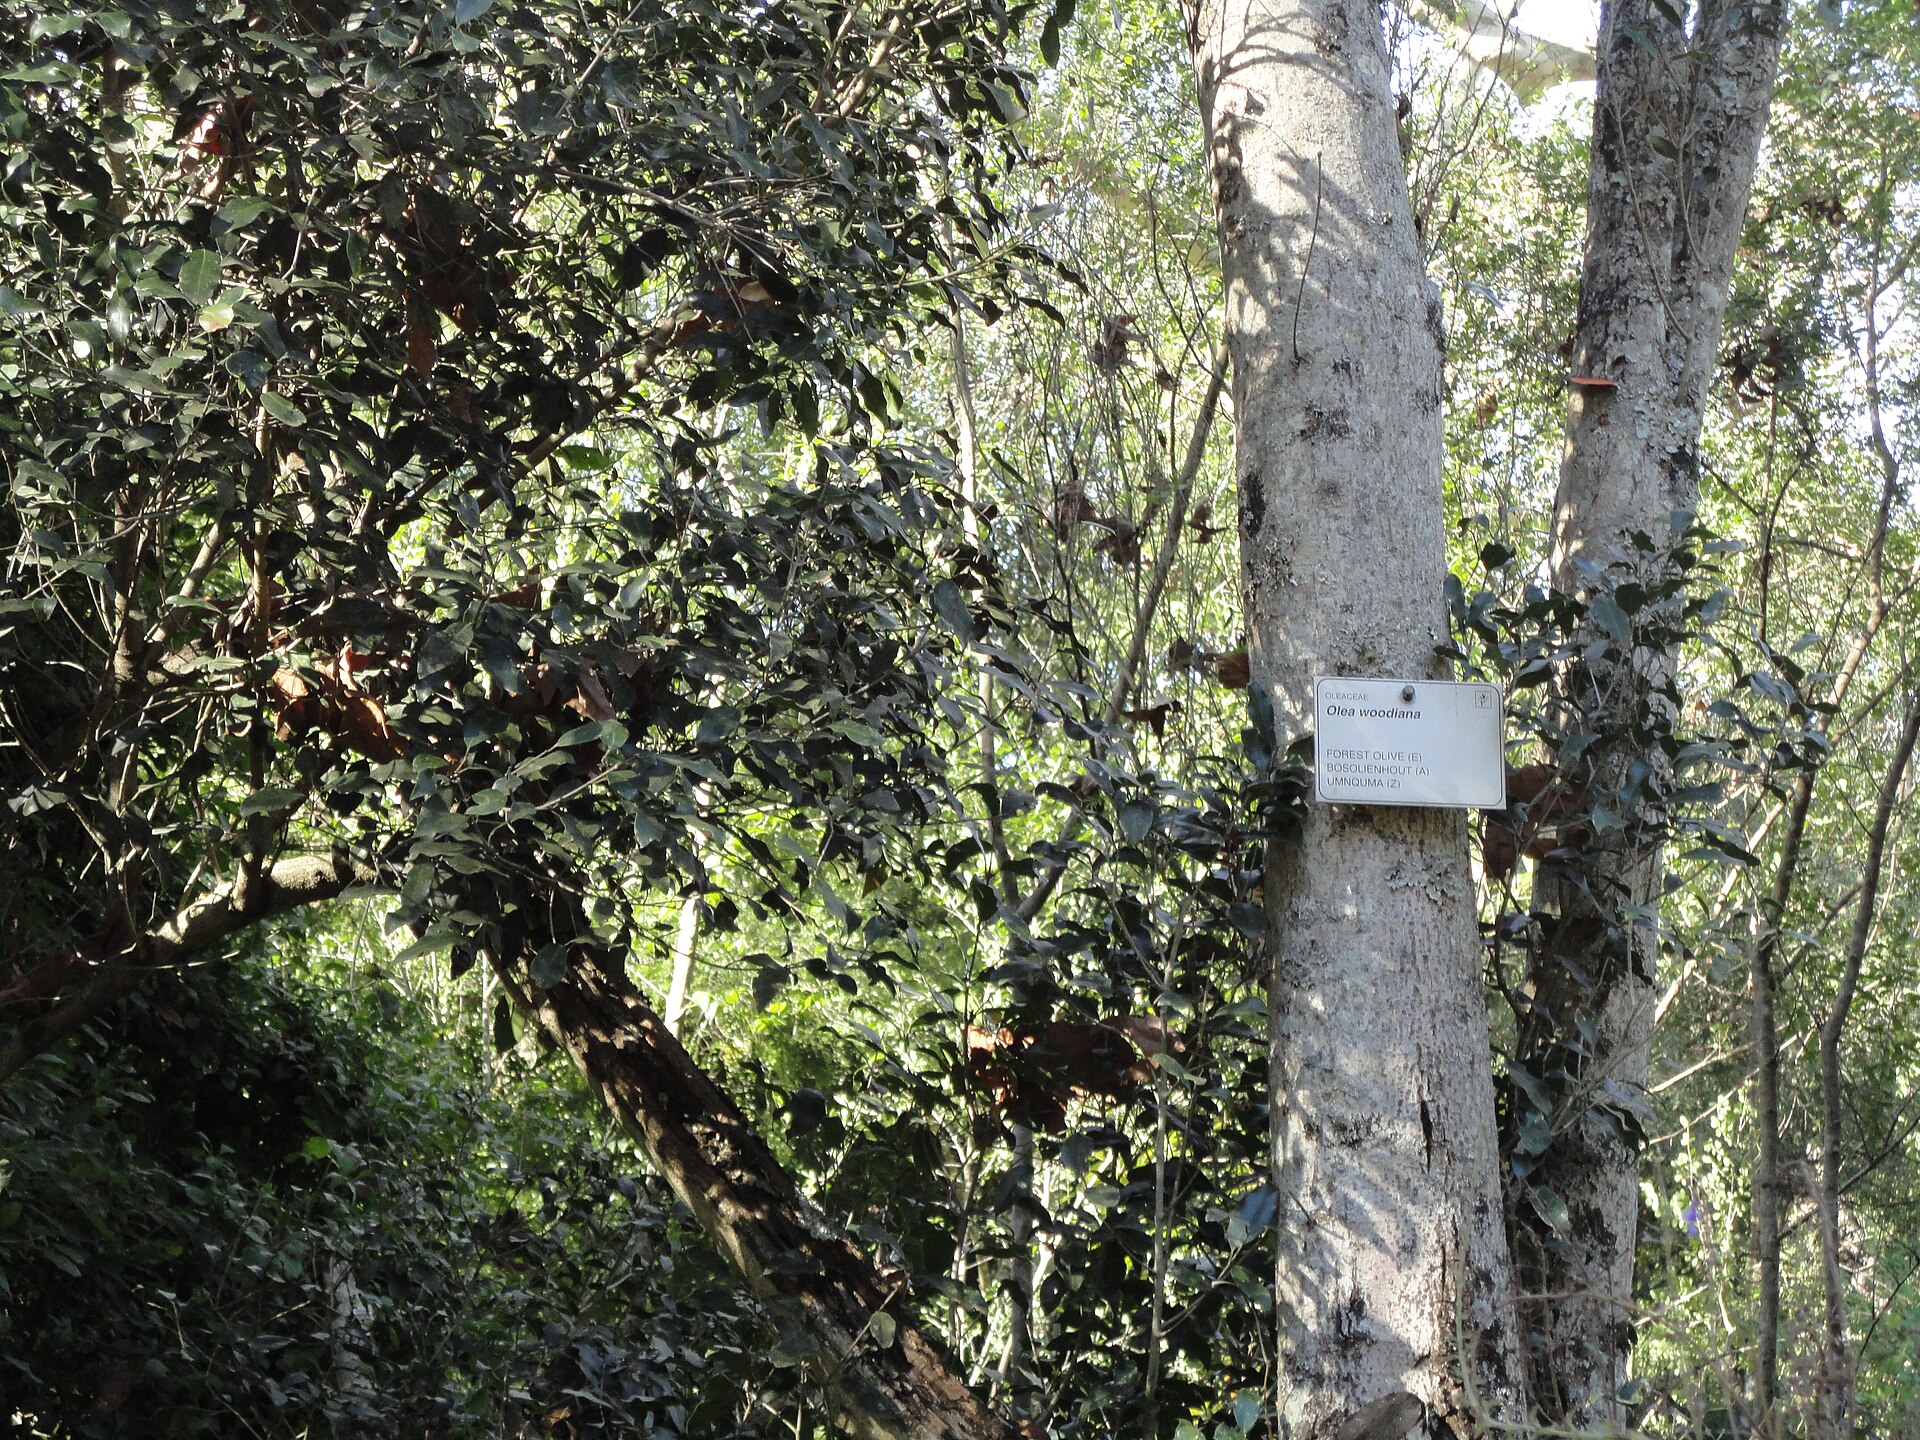
native Olia woodiana in forest of Kwa-Zulu-Natal, South Africa. Photo by MJK via Wikimedia

The forests of the Southern Hemisphere faces an elevated risk from introductions of tree-killing arthropods and pathogens. I have already blogged about individual threats to the trees of South Africa, Australia, South America, and Madagascar. This blog will add information about those invasions and provide an overview and call for action.

Burgess and Winfield (2026) [full citation at the end of this blog] – eminent pathologists from South Africa – warn their colleagues that the economic and biological barriers that have long protected the biomes of the Southern Hemisphere from bioinvasion have now collapsed. While these countries remain geographically distant from each other and the Northern Hemisphere, and their floras are certainly still unique, they are now participating in global trade. In addition, they increasingly rely on industrial plantation forestry dominated by non-native tree species – some of them from the North. Finally, climate change is putting additional stress on all these systems.

Burgess and Winfield (2026) advise their colleagues to learn lessons from the alarming history of bioinvasion in the Northern Hemisphere. Over the past century, these forests have been battered by a series of invasions by tree-killing pathogens. They mention the examples we know too well: chestnut blight (Cryphonectria parasitica), white pine blister rust (Cronartium ribicola), “Dutch” elm disease (Ophiostoma ulmi/Ophiostoma novo-ulmi), pine wilt nematode (Bursaphelenchus xylophilus), sudden oak death (Phytophthora ramorum), ash decline (Hymenoscyphus fraxineus), laurel wilt (Harringtonia lauricolia), ʻōhiʻa or myrtle rust (Austropuccinia psidii), https://www.dontmovefirewood.org/pest_pathogen/ohia-rust-html/ and rapid ʻōhiʻa death (Ceratocycstis lukobia and huliohula). They do not address the similarly depressing history of arthropod interchanges among these realms.

Burgess and Winfield (2026) warn that these invasions are not anomalies but rather predictable outcomes of global commerce – especially in “plants for planting” – interacting with the ecological vulnerability arising from the biogeographic similarity of these temperate and boreal forests. The Northern Hemisphere is dominated by a single flora (the Holarctic).

The Southern Hemisphere has an astounding seven floral kingdoms, distributed as follows: Chile-Patagonian, Neotropical, African, Indo-Malesian, Australian, Novozealandic, and Cape. These regions were formerly part of Gondwanaland. Each has an exceptionally high level of endemism (Burgess and Wingfield 2026), but with phylogenic relationships to the flora of other regions. Changing trade patterns are opening introductory pathways for exchange of tree pests hosted by related but geographically distant species. The regional floras’ uniqueness multiplies the conservation importance of protecting them. I summarize Southern Hemisphere countries’ levels of endemism at the end of this blog.

The lessons Burgess and Wingfield (2026) draw from the bioinvasion history of the Northern Hemsphere include:

1) Trade in living plants – and even seeds – creates a high risk that accompanying microbes will be introduced. As noted by others – e.g., Tanney et al. (2025) – members of each plant species’ “phytobiome” are ubiquitous, diverse, difficult to detect, and sometimes capable of causing serious diseases, especially in naïve hosts.

2) After introduction, these microbes can evolve rapidly to adapt to new environments or hosts. They often become more aggressive and difficult to manage in the process. Plant health officials need to anticipate this evolution.

3) Impacts can be catastrophic when a dominant tree species is killed. When chestnut blight killed the vast majority of chestnut trees in North America it destabilized ecosystems and reshaped successional trajectories.

4) The threat is magnified when the receiving ecosystem is a forestry plantation because of the extensive monocultures.   

Building on Burgess and Wingfield (2026) and other sources (where noted), I provide the following summary of threats to native and planted forests in these regions. Some, e.g., Phytophthora cinnamomi and Sirex noctilio, were introduced many decades ago. But too many are recent arrivals.

I. Threats to tree species native to the region.

1) Australia

trees killed by Phytophthora cinnamomi; photo by Western Australia Parks & Wildlife
  • Carnegie et al. (2026) report that more 300 non-native insect pests, pathogens and nematodes are established on tree or shrub hosts in Australia. Twenty percent have caused moderate to high impacts to commercial plantations, urban forests, or trees in natural ecosystems.
  • Phytophthora cinnamomi: As noted, this pathogen was introduced decades ago. It has devastated jarrah (Eucalyptus marginata) forests and diverse plant communities. It causes severe mortality in Proteaceae, Epacridaceae, and Fabaceae. Of ~5700 described plant species in the state of Western Australia, 40% ( >2,300) can be killed (Carnegie et al. 2026).
  • Austropuccinia psidii (myrtle rust): threatens trees in the Myrtaceae worldwide. The rust has spread widely recently, causing severe ecological impacts in invaded regions. The “epidemic strain” introduced to Australia (and other regions) does not infect the commercially important genus Eucalyptus, which probably explains Australian authorities’ lackluster response. However, other lineages of the pathogen found in South America do infect Eucalyptus; introduction of one of these to Australia could be disastrous. Cautionary example of how rapidly a plant pathogen can conquer new ecosystems (Burgess and Wingfield 2026). Already, plant 76 species have been determined to be at risk to myrtle rust. The early focus has been on understory species in the eastern rainforests. Now that myrtle rust has been detected in Western Australia, a biodiversity hotspot with more than a thousand Myrtaceae taxa, most of which are expected to be susceptible. [Summary of Proceedings: Australian Myrtle Rust Conference Sydney, June 2023]
  • Polyphagous shot hole borer Euwallacea fornicatus s.s. (PSHB) and associated pathogen F. euwallacea were detected in 2021, probably three years after it established in Western Australia. Nearly 9% of hosts are regionally indigenous species, 21.3% native to other parts of the continent. There will probably be a considerable impact on the health of conservation reserves & national parks in the future. After trying for four years to eradicate the population, in November 2025, the National Management Group began a transition to a Management Response Plan. This new approach will impose significant additional expenses on local governments and communities for tree removal and replacement (Dell, Xu, & Chi 2026). Meanwhile, the state of New South Wales (2,000 miles away on the other side of the continent) initiated surveillance for PSHB. An assessment determined that 47% of urban trees in Sydney are susceptible to PSHB (Carnegie et al. 2026).
  • Erythina gall wasp Quadrastichus erythrinae (Carnegie and Nahrung 2019). Although Australia is home to at least one native species in the Erythrina genus, E. vespertilio, this pest has not been included on the environmental pest watch list. 

2) New Zealand

native forest on North Island, New Zealand, with kauri tree; photo by F.T. Campbell
  • Kauri dieback / Phytophthora agathidicida is killing Agathis australis, a keystone species that shapes forest structure and has enormous cultural importance for the Maori.

3) South Africa

  • Phytophthora cinnamomi — in the country since 1931 — threatens ecosystem collapse in Cape Floral Kingdom (Burgess and Wingfield 2026).
  • Polyphagous shot hole borer Euwallacea fornicatus s.s. and associated pathogen F. euwallacea The largest outbreak of Fusasrium disease in the world: it is present in every province except Limpopo. The Disease is recorded on 162 tree species. Seventy-eight of these species are indigenous to the country. Eighty-four are “competent” hosts and 78 are “Fusarium colonised” hosts (Townsend, Hill, Hurley and Roets 2025).
  • Fungus Seiridium neocupressi detected on the native tree, Widdringtonia nodiflora year The two other species in the genus, W. wallichii and W. schwartzii, occur in small endemic and threatened populations (Wingfield et al. 2022).

4) Madagascar

  • Leptographium calophylli killing an endemic tree species in mid-level elevation humid and subhumid forests, Calophyllum paniculatum.  

5) South America

  • Polyphagous shot hole borer Euwallacea fornicatus s.s. and associated pathogen F. euwallacea has been detected in Brazil, Argentina, and Uruguay. Dell, Xu, & Chi (2026) report that in Uruguay a significant number of native species are reproductive hosts for the beetle. Models developed by Coates and Philips (2026) indicate PSHB could thrive in more suitable habitats.
  • One of the continent’s native conifers, Austrocedrus chilensis is under attack by both an introduced aphid, Cinara cupressi and the pathogen Phytophthora austrocedri
Chilean cypress; photo by LBM via Wikipedia

Lantschner et al. (2026) identified seven independent introduction events of E. fornicatus: to the continental U.S., Hawai`i, South America, Central Europe, Spain, Türkiye, & South Africa.

II. Threats to plantations:

1) Co-evolved insects and pathogens have followed their Pinus hosts to plantations in the Southern Hemisphere due to biosecurity failures

  • Insects: Sirex noctilio (decades ago); recently Sirex obesus in Brazil (2023); Orthotomicus erosus and Cyrtogenius luteus (Stazione, Soliani, and Cognato 2026).
  • Pathogens: Fusarium circinatum, Dothistroma septosporum, Diplodia sapinea,  Phytophthora pinifolia, Lecanosticta acicula.

2) Because the Myrtaceae family is distributed around the Southern Hemisphere, plantations of Eucalyptus trees are now being damaged by both pathogens from their native Australian range (Teratosphaeria spp.) and local pathogens that have switched hosts (Chrysoporthe cubensis and Chrysoporthe deuterocubensis).

Burgess and Wingfield (2026) express fear that another set of pathogens, rapid ohia death (Ceratocystis lukuohia and Ceratocystis huliohia) might spread from Hawai`i farther across Oceania to New Zealand and other locations with important species in the Metrosideros genus. I note that the more virulent (on ʻōhiʻa) C. lukuohia belongs to an Asian-Australian clade (Luiz et al. 2023).  

Australia

I blogged in November 2022 about how surprising tardy Australia was in implementing phytosanitary programs to protect the nation’s forests. Scientists had spent 30 years trying to get such a program implemented. Burgess and Wingfield (2026) point out that 16 of 17 pathogens detected in Australia over the period 1996 – 2017 had established; several had had major impacts. None has been eradicated. They also note that the introduction of Austropuccinia psidii exposed significant weaknesses in post-border surveillance and response. 

The Australian federal govt has implemented a detection trapping program targeting the Asian spongy moth (= flighted spongy moth complex) at the 4 major ports (i.e., Melbourne, Hastings, Geelong and Portland) since 1996.

Carnegie et al. (2026) describe some helpful steps. They focus on establishment in 2022 of a National Forest Pest Surveillance Program (now called Forest Watch Australia). The program is funded by a levy on forest plantation growers and State governments, based on the relative risk to each region. Surveillance efforts are concentrated in areas deemed high risk areas for entry and establishment of forest pests. Program is coordinated through the federal agency, Plant Health Australia. It provides professional training for surveillance and diagnostic staff on an annual basis. Staff also conduct risk modelling and analysis to identify high-risk areas for surveillance in all major capital cities — Sydney, Melbourne, Brisbane, Hobart, Adelaide, Perth and Darwin.

The Australian program encounters the universal challenges regarding sustained resources, the diagnostic burden placed on scientists, and ownership of data. Carnegie et al. (2026) and Burgess and Wingfield (2026) discuss the growing availability of new tools for detection, e.g., molecular diagnostic tools.

Response options are guided by the national Emergency Plant Pest Response Deed and PlantPlan,  which outlines agreed government and industry responsibilities and cost-sharing protocols.  

Carnegie et al. (2026) praise especially the sentinel tree component of the surveillance program. Participants include governments at the federal, state, and municipal levels; botanical gardens; and industry. In 2024/25, trained staff inspected 5,136 trees of more than 50 species across 45 genera nationwide. Thanks to this expanded effort, the detection rate of new species has doubled since 2018, from ~ 1.5 to ~ 3 / year. Still, in three of four cases discussed by Carnegie et al. (2026), the introduced organisms were determined to be too widespread for eradication to be successful. They cite the PSHB outbreak in Perth as an example. Carnegie et al. (2026) advocate strengthening sentinel tree surveillance in urban landscapes so detection will occur sufficiently early to allow consideration of initiating an eradication or containment response. One worrisome aspect: there is no requirement to conduct more thorough surveillance or diagnostics on a species detected in the country once it has been ruled not “of concern”.

Burgess and Wingfield (2026) advocate embracing broader preventative approaches that address the underlying mechanisms of pathogen emergence and spread. I forthcoming blog will discuss proposed new approaches.

Background: Southern Hemisphere Flora

South Africa

As I blogged recently, South Africa’s flora is diverse (more than 20,000 indigenous species) and has high levels of endemism. That blog did not discuss the Myrtaceae family – my focus now because of the spread of the pathogen Austropuccinia psidii. According to Braam van Wyk and Hugh Glen (pers. comm.), the country has 24 native Myrtaceous species. These include 14 species in the Eugenia genus, six in the Syzygium genus. The one Metrosideros grows in the Cape Floristic Region. All the others occur in forest or grassland along the Indian Ocean Coastline well into Mozambique and further inland – some into Botswana and Zimbabwe.

Australia                      

Australia ranks second on Earth in the proportion of its flora that is endemic: 88% of plants. Australia comprises the native range of 38% of all Myrtaceae species on Earth, and of 66% of genera in the family (Brett Summerell, 2023 workshop). These 87 or 88 genera contain ~ 2,250 species and subspecies (Makinson 2018). This plant family constitutes ~10% of the continent’s native flora. They occur in 11 of 13 major vegetation formations (Carnegie et al.2026). The southwestern corner of Western Australia alone has ~5700 described plant species (Carnegie et al 2026).

Rhodomyrtus psidioides – one of the Australian Myrtaceae under greatest threat from myrtle rust; photo by Zaadero via Wikimedia

The island of Madagascar is home to 12,000 plant species, of which 83% are endemic.

SOURCES

Burgess T.K., and M.J. Wingfield. 2026. Unveiling a Hidden Menace: Invasive Tree Pathogens, Less Known but Increasingly Threatening Southern Hemisphere Forests Annual Review of Phytopathology #s

Carnegie AJ, Summerell BA, Trollip C, Tovar F, Smith DI and McDonald J (2026) Sentinel trees for early detection of non-native forest pests and pathogens in AU. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Ceriani-Nakamurakare, E., Johnson, A.J. and Gomez, D.F. (2023) Uncharted Territories: First report of Euwallacea fornicatus (Eichhoff) in South America with new reproductive hosts records. Zootaxa, 5325 (2), 289–297. https://doi.org/10.11646/zootaxa.5325.2.10

Lantschner, M.V., Ceriani-Nakamurakare, E., Johnson, A.J. et al. Invasion history reconstruction and potential distribution of the ambrosia beetles Euwallacea fornicatus and E. perbrevis, two global emerging pests. J Pest Sci 99, 100 (2026). https://doi.org/10.1007/s10340-026-02070-w

Luiz, B.C., C.P. Giardina, L.M. Keith, D.F. Jacobs, R.A. Sniezko, M.A. Hughes, J.B. Friday, P. Cannon, R. Hauff, K. Francisco, M.M. Chau, N. Dudley, A. Yeh, G. Asner, R.E. Martin, R. Perroy, B.J. Tucker, A. Evangelista, V. Fernandez, C. Martins-Keli’iho.omalu, K. Santos, R. Ohara. 2023. A framework for establishlishing a rapid ‘Ohi‘a death resistance program  New Forests 54, 637–660. https://doi.org/10.1007/s11056-021-09896-5

Stazione, L., Soliani, C., Cognato, A. et al. Reconstructing the invasion history of the bark beetles Orthotomicus erosus and Cyrtogenius luteus (Coleoptera, Curculionidae, Scolytinae) in South America. Biol Invasions 28, 49 (2026). https://doi.org/10.1007/s10530-026-03779-6

Tanney, J.B., M. Kemler, M. Vivas, M.J. Wingfield, and B. Slippers. 2025. Silent invaders: the hidden threat of asymptomatic phytobiomes to forest security. New Phytologist (2025) 247: 533–545 doi: 10.1111/nph.70209

Wingfield, M.J. S. Marincowitz, N.Q. Pham, F. Roets, T. Paap, B.D. Wingfield, J. Aylward. 2022. Cypress canker: An important disease discovered for the first time on a native South African tree. Plant Pathology 2022;71:1735-1742

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Update on invasive plants in Hawai`i

Cibotium glaucum in Hawaii Volcanoes National Park; F.T. Campbell

A year ago I blogged about the status of Hawaiian species in the face of high levels of bioinvasions. I now update that discussion as it pertains to one of the invaders, the Australian tree fern Sphaeropteris cooperi.

S. cooperi has successfully invaded multiple regions, including the southern coast of South Africa, the Azores and Mascarene Archipelagos, and Hawai`i. The invasion’s impacts have been assessed only in Hawai`i. Studies found that the non-native tree ferns have outcompeted the dominant native tree fern Cibotium glaucum (Cibotiaceae), and altered leaf litter composition hence soil nutrient cycling. This in turn affects species assemblages (van den Berg et al. 2025).

Chau, Walker and Mehltreter (2013) documented the litter and soil chemistry in Hawaiian rainforests. They found that S. cooperi produces more leaves that grow faster, contain more nitrogen and phosphsorus, and decompose faster than the leaves of the dominant native tree fern C. glaucum. They compared the effect of leaf litter from the native and tree ferns on the growth and nutrient content of four native angiosperm species when they were grown in N-rich forest soil and P-rich landslide soil. The results suggested that nitrogen availability is the strongest driver of growth. The introduced tree fern, S. cooperi, can thus prompt more rapid growth of some native HI plants. They point out, however, that under natural conditions, native plants must compete for these additional nutrients with various non-native plants, including S. cooperi. The ultimate impact, then, remains unclear.

van den Berg et al. (2025) report that other invaded sites are at great risk Both the Garden Route region of South Africa and La Reunion Island in the Mascarene Archipelago in the eastern Indian Ocean have high bioidiversity. Both contain large, globally-recognized protected areas established to protect the native biodiversity: UNESCO Garden Route Biosphere Reserve and Reunion National Park. Despite their biological importance, both are among the top10 most invaded countries/territories globally (Tuberlin et al. 2017).

Sphaeropteris cooperi; photo via Easyscape

While climate change is expected to reduce the extent of suitable habitat for the Australian tree fern in both South Africa and La Reunion, the current situation is troubling. At present the tree fern occupies a narrower range of climatic conditions in both the Garden Route and especially on La Reunion than in Australia. (On La Reunion, 13.74 % of the fern’s apparent niche remains unoccupied.) van den Berg et al. (2025) are not sure what factors might be limiting the tree fern’s spread. They do urge educational campaigns to persuade people living near the Biodiversity Reserve to avoid planting the non-native tree fern.

The tree fern’s actual niche is somewhat uncertain because predation by deer (non-native to Australia) might have reduced its reproduction. The authors mention this but do not speculate further on the possible response of the fern to the absence of such stresses on La Reunion.

SOURCES

Chau, M.M., Walker, L.R. and Mehltreter, K. An invasive tree fern alters soil and plant nutrient dynamics in Hawaii. Biol Invasions 15, 355–370 (2013). https://doi.org/10.1007/s10530-012-0291-0

Turbelin,A.J., Malamud,B.D., Francis,R.A. 2017. Mapping the global state of invasive alien species: patterns of invasion and policy responses. Glob. Ecol. Biogeogr. 26,78–92. https://doi.org/10.1111/geb.12517.

van den Berg, M.L., G. Singh, E.J. McCulloch-Jones, M. Rouget, D.M. Richardson, T.B. Robinson. 2025. The invaded range of the tree fern Sphaeropteris cooperi is predicted to shrink in two southern hemisphere biodiversity hotspots. African Journal of Botany 178 (2025) 390-399

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
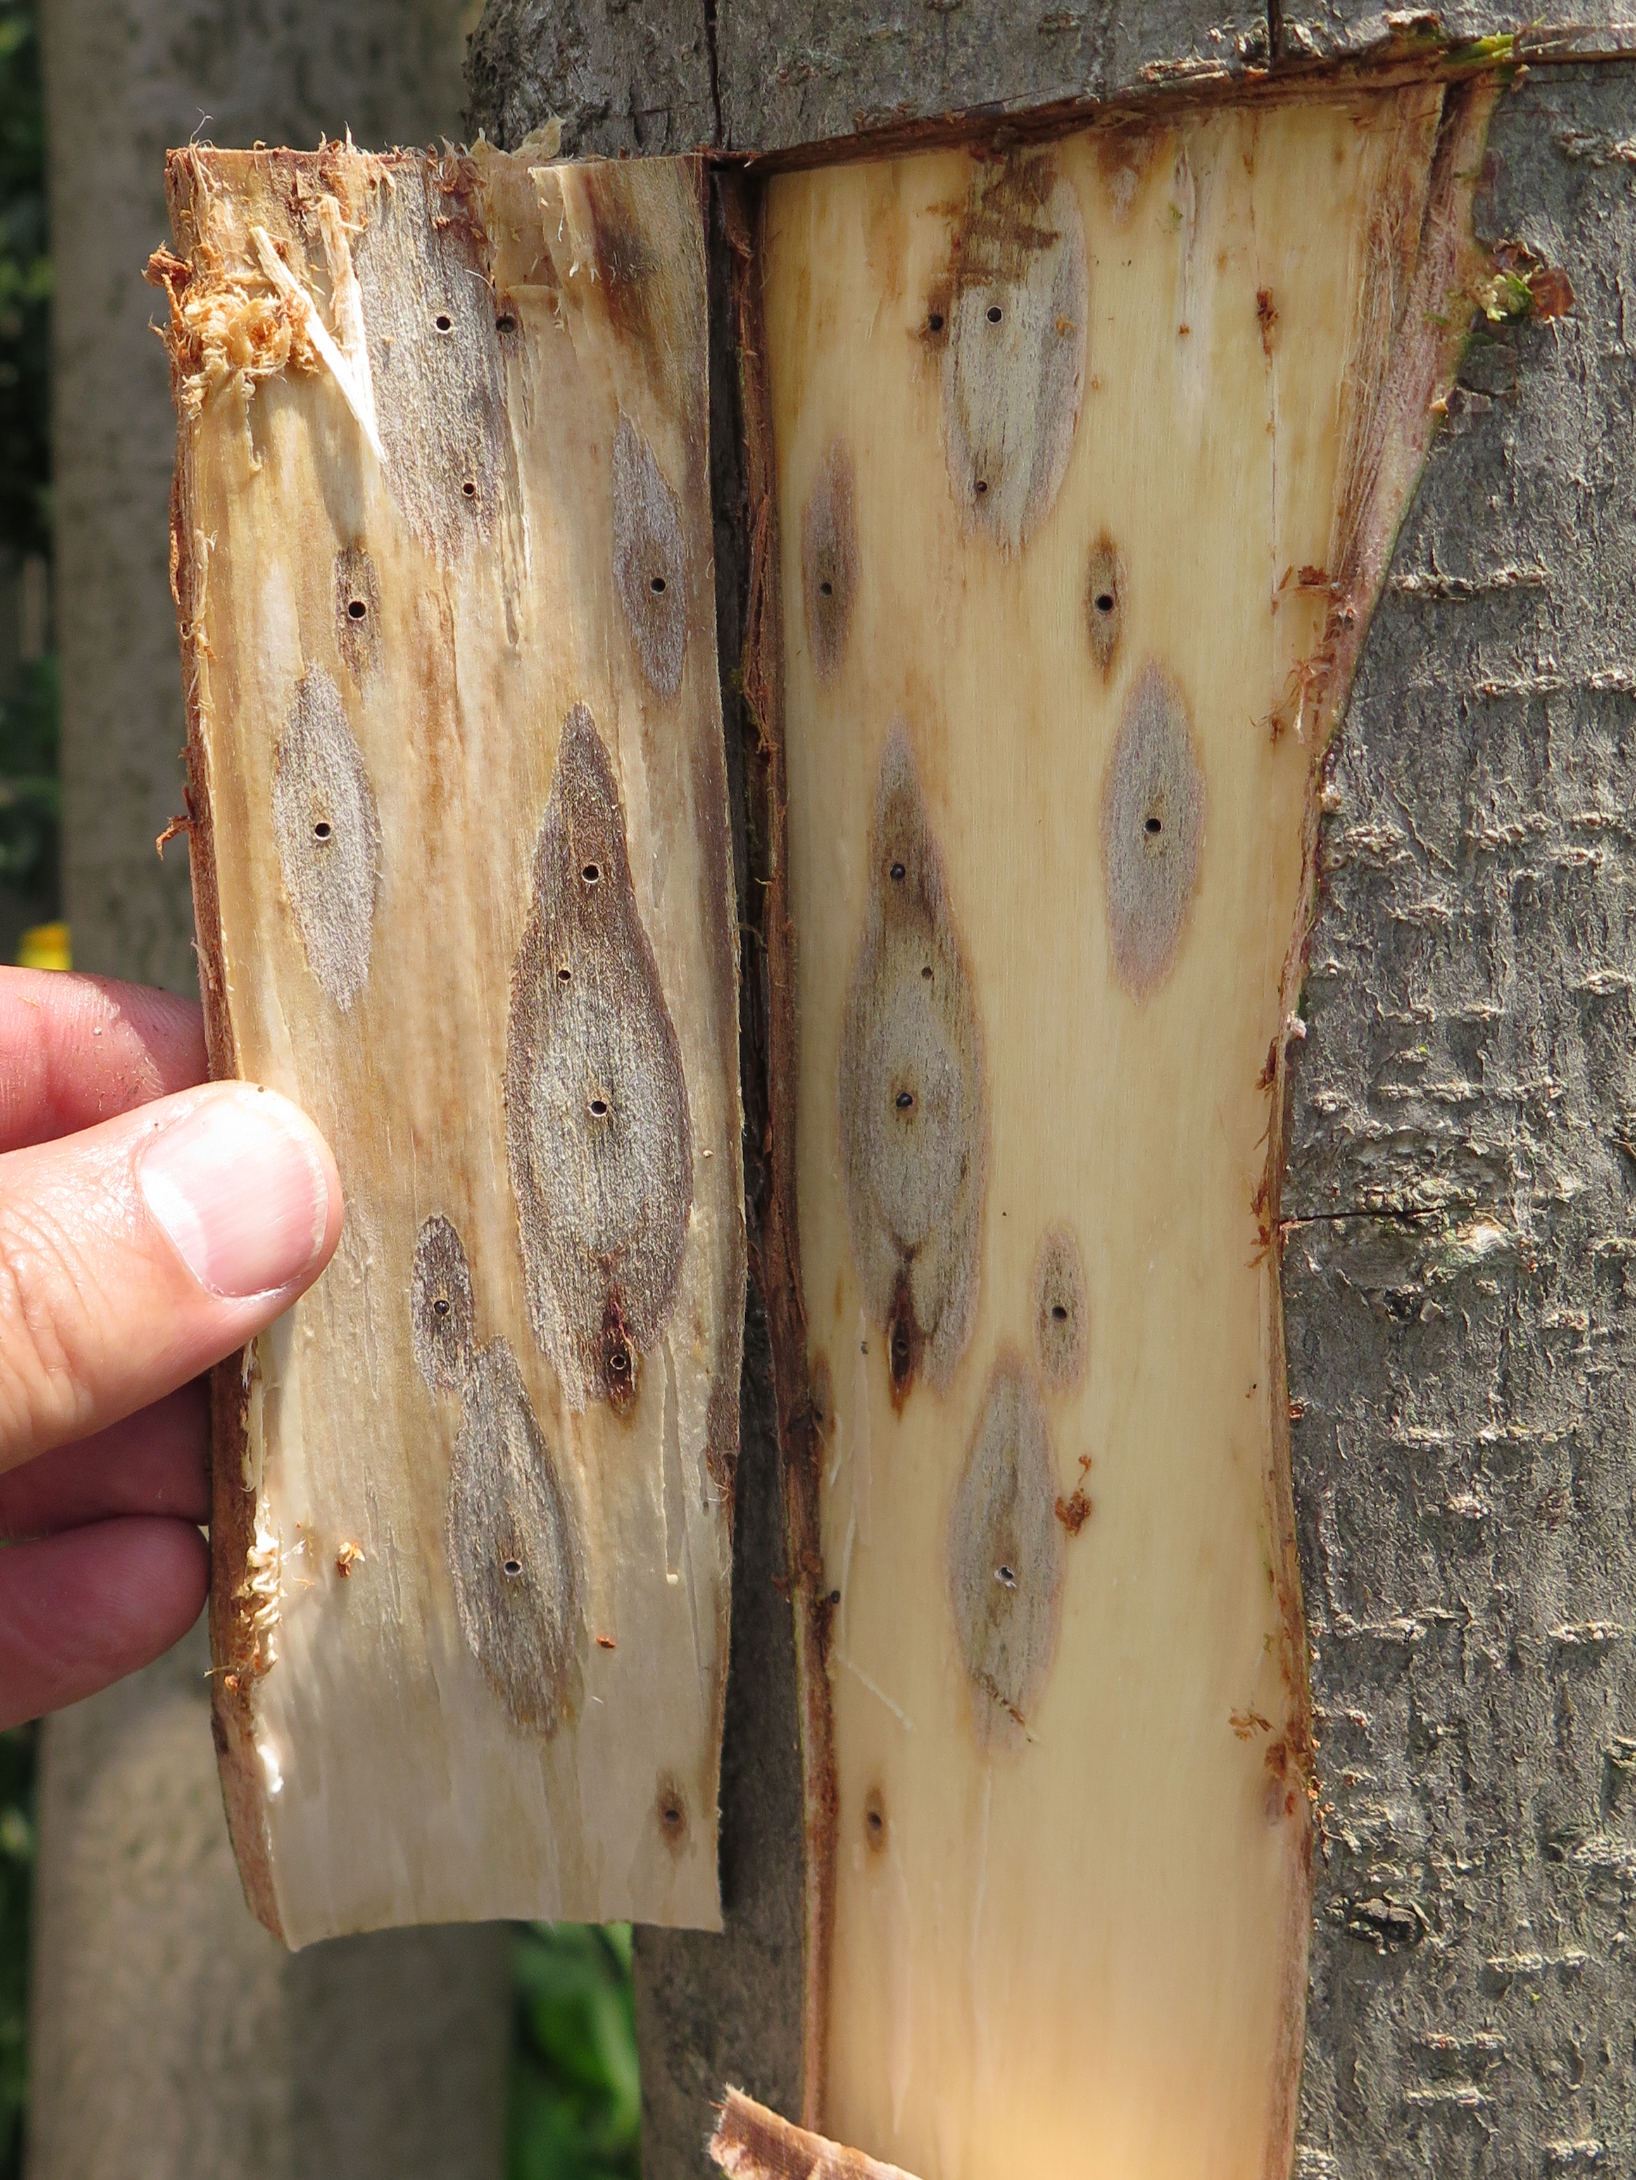
https://fadingforests.org

Invasive species on the African Continent

We are beginning to get more information about invasive species on the African continent.

a flyer naming principal invasive ornamental plants in Kruger National Park

In several countries, the focus has been on threats to agriculture. Previous blog about horizon-scanning in Ghana. In Zimbabwe, N. Mudada and colleagues (2026; full citation and the end of this blog) found alarming, if not surprising, levels of risk to food production from introduced invasive plants. They investigated 1,668 human-aided transboundary plant introductions at 14 ports of entry and non-official crossing points over the course of four years.

They estimate that the 20,000 trucks that transported maize into the country over the four years carried over 20,700 metric tons of weed seeds and rubbish! They recorded detections of 11 species in eight orders. The pathways are familiar. As noted, several weeds were contaminants of grain shipments; Convolvulus arvensis in wheat for human consumption, Helianthus annus and Datura stramonium in maize for animal feed. Adenium obesum and Vitex agnus-castus were being smuggled for planting as flowers and ornamentals. (Vitex agnus-castus was also smuggled in passenger baggage for its medicinal properties). Several Lemna species (an aquatic plant) were also smuggled for planting as animal feeds.

In some cases, the focus is the threat to native ecosystems. I posted a blog the about threat of an introduced pathogen to trees in the remnant rain forests of Madagascar.

South Africa still has the lead in addressing invasive species. Regarding invasive plants specifically, the country has the benefit of more than 150 years of botanizing. The richness of the region’s flora is globally recognized. South Africa also has a long history of studying and managing invasive species, especially plants.

South African scientists and colleagues in Botswana, Eswatini, Lesotho, and Namibia have published four editions of the Flora of the Southern Africa region since 1984. In 2006, the PRECIS database of the South African National Biological Diversity Institute (SANBI) was combined with the Tropical African Plant Checklist published by the Conservatory and Botanical Garden of Geneva to create the African Plant Checklist and Database Project. It is continually updated. This is the first continental flora checklist for Africa; it fulfils countries’ obligations under the Convention on Biological Diversity’s Global Strategy for Plant Conservation.

For South Africa specifically, scientists have produced a national plant checklist that is updated annually.

The 2025 Checklist reports that 21,539 plant species are extant outside cultivation in the country; these comprise 20,204 indigenous species and 1,329 naturalized species. Thus, 6% of the total flora is non-indigenous. Of these, 649 (48.8% of the non-indigenous species, 3% of all plants) of them are invasive.

[Naturalized species are defined as species whose documented natural range does not include South Africa, but have overcome a biogeographic barrier and now sustain self-replacing populations for two or more life cycles or over a given period of time in the country. These populations are maintained without direct intervention by people, or despite human intervention. Invasive species meet the above definition plus produce reproductive offspring, often in large #s at considerable distances from the parent and/or site of introduction, and have the potential to spread over long distances.]

Since the previous checklist was published in 2006, botanists have identified 1,048 additional species – a 4.9% increase. Eighty-two percent of the newly identified species (865 species) are “naturalized”. Specifically, 414 new species are categorized as naturalized (a 31.1% increase), and 451 new species are classified as invasive (a whopping 69.5% increase). Le Roux and Klopper attribute these steep increases to active botanizing by SANBI’s Invasive Species Programme (begun in 2008), and the Southern African Plant Invaders Atlas Project (begun in 2010).

Of the 384 plant families present in South Africa, 350 contain at least some indigenous species. Thirty-four families contain only naturalized species. Among the 2,189 plant genera present, 459 (21%) contain only species that are non-indigenous.

Three families stand out because of the particularly high numbers of naturalized species: Fabaceae (143 species; 11% of all naturalized species), Asteraceae (140 species; 10%), Poaceae (123 species; 9%). Two of these families — Asteraceae and Fabaceae — are also the largest families among native South African plants. The third, grasses (Poaceae), ranks seventh in the list of most specious families indigenous to South Africa. The next group of families with high numbers of naturalized species has less than half as many invasive species: Myrtacae (55), Amaranthacea (52), Solanaceae (48). None of these families ranked within the top 20 families of indigenous plant species.

The genera with the most naturalized species were Solanum, Euphorbia and Acacia (all 24 or 23 species).

Acacia cyclops; photo by David M. Richardson

South African scientists are also exploring how to balance conflicting goals and perspectives when an invasive plant species has economic or social value. The example chosen by Mbobo et al. (2025) is guava (Psidium guajava) – a nutritious and popular tropical fruit grown commercially in South Africa, but also invasive along roadsides, watercourses and forest margins. Invasions are especially common in eastern parts of country; large monocultures are found in KwaZulu-Natal. Outbreaks have also been detected at five sites in Western Cape in riparian zones and at a hot spring. Mbobo et al. (2025) note that the microclimatic conditions at this last location differ from the broader conditions in the region – which are what most models would measure.

The scientists used models to predict where guava might invade – especially in large monocultures – and compared those areas to where the tree can be grown in cultivation with human inputs, e.g., irrigation. They then assessed whether six regulatory approaches would avoid restricting guava farming in areas at minimal or low risk while still protecting vulnerable locations. They also considered the amount of information required to implement the approach and costs of acquiring the information; and level of likely public acceptance. Mbobo et al. (2025) laid out the trade-offs between continuing to regulate planting of the species at the provincial level vs. at the municipal level. Prohibiting planting of guava in provinces where it is recorded as invasive allows some plantings near natural forests and riparian areas that are highly susceptible to guava invasions. On the other hand, nearly half of the prohibited area is outside the known or likely at-risk area. The provinces do allow exceptions through a permit process. Adopting more geographically limited rules by regulating at the municipal level would enable a tighter link to geographic areas at highest risk. However, this approach does not address long-distance seed dispersal by animals. Furthermore, the very detailed regulations might confuse stakeholders and complicate enforcement. Also, the models lack sufficiently fine spatial resolutions to predict invasible areas so accurately. Finally, the reduction in regulated area is minimal (~ 14%), so the economic benefits are unlikely to outweigh the significantly higher administrative costs and risk of allowing guava invasions in new sites.

Guava fruit on tree; Roenashy via Wikimedia

Gildenhuys et al. (2026) analyzed the factors that drive which non-native plants establish where. They assessed the roles of temperature, precipitation, urbanization intensity, urban area, travel time, year of city’s establishment, and human population density in determining which plant species are present in 54 urban centers in Western Cape Province. The cities have significant differences in climate: Mediterranean in the far southwest, warm temperate in the southeast, and semi-arid towards the interior. The expectation was that these drivers and assembly processes are influential at more advanced invasion stages when the species have already overcome some barriers to dispersal, so are now found in reasonably suitable habitats.

Gildenhuys et al. (2026) found temperature and precipitation were most important in determining plant species’ presence. This was especially true at the boundary between arid and mesic climates. These strong environmental gradients are the same ones which have driven high differences in native species presence across the province. [See pamphlet describing invasive plants in Cape Town.] This finding supports the “Goldilocks hypothesis”: that non-native plant species assemblages are driven by the same abiotic variables as native species assemblages. While did not directly study the “Biome decides hypothesis” (the composition of non-native flora is mediated by the biotic effects of native flora and fauna), Gildenhuys et al. (2026) doubt its applicability here because native species’ presence has probably been greatly reduced by the effects of urbanization.

Urbanisation intensity itself ranked third as a factor. Its effect was strongest at low to medium urbanization intensities. Because urbanization creates novel habitats, such as, “hardscapes” of paved surfaces that resemble deserts, their non-native plant assemblages are dominated by similar, urban specialist, species. At lower urbanization intensities a greater variety of habitats is available. Gildenhuys et al. (2026) conclude that urbanization acts primarily as a driver of opportunistic habitats for species at later invasion stages rather than as a filter of species introduction.

An earlier study found a similar effect from road density (often associated w/ urbanization) as an explanation for where specific woody non-native species establish. They do concede that larger urban areas might experience greater propagule pressure.

Gildenhuys et al. (2026) note that recent globalization of the plant trade has probably changed the specis planted in urban centers. For example, cities in the Western Cape are increasingly replacing English oak (Quercus robur) with more disease-resistant oaks. The change might reflect greater environmental awareness and regulations issued under the National Environmental Management: Biodiversity Act 10 of 2004. In newly established urban centers, fewer invasive species are being planted — at least among trees.

SOURCES

Gildenhuys, C.P., L.J. Potgieter, C. Hui, D.M. Richardson. 2026. Drivers of compositional turnover of the NIS urban flora in the W Cape, South Africa. Urban Ecosystems (2026) 29:51 https://doi.org/10.1007/s11252-026-01919-3

Le Roux, M.M., R.R. Klopper. 2025. Taking stock of South Africa’s flora. South African Journal of Botany 184 (2025) 571-579

Mbobo, T., D.M. Richardson, A. Datta, K.T. Faulkner, J.R.U. 2025. Wilson. Spatially-Differentiated Reg of NIS Can Be Improved Using Spp Distribution Models: Psidium guajava in South Africa as a Case Study. Diversity and Distributions. 2025 31:e70102 https://doi.org/10.1111/ddi.70102

Mudada, N., J. Chitamba, E. Nyangani, C. Chapano, N. Mapope,and W. Ngezimana. 2026. Weeds associated with cross border traffic, their approach and infestation rates in Zimbabwe.  ISABB Journal of Food and Agricultural Sciences. Vol. 12(1) January-June 2026. DOI: 10.5897/ISABB-JFAS2025.0192

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
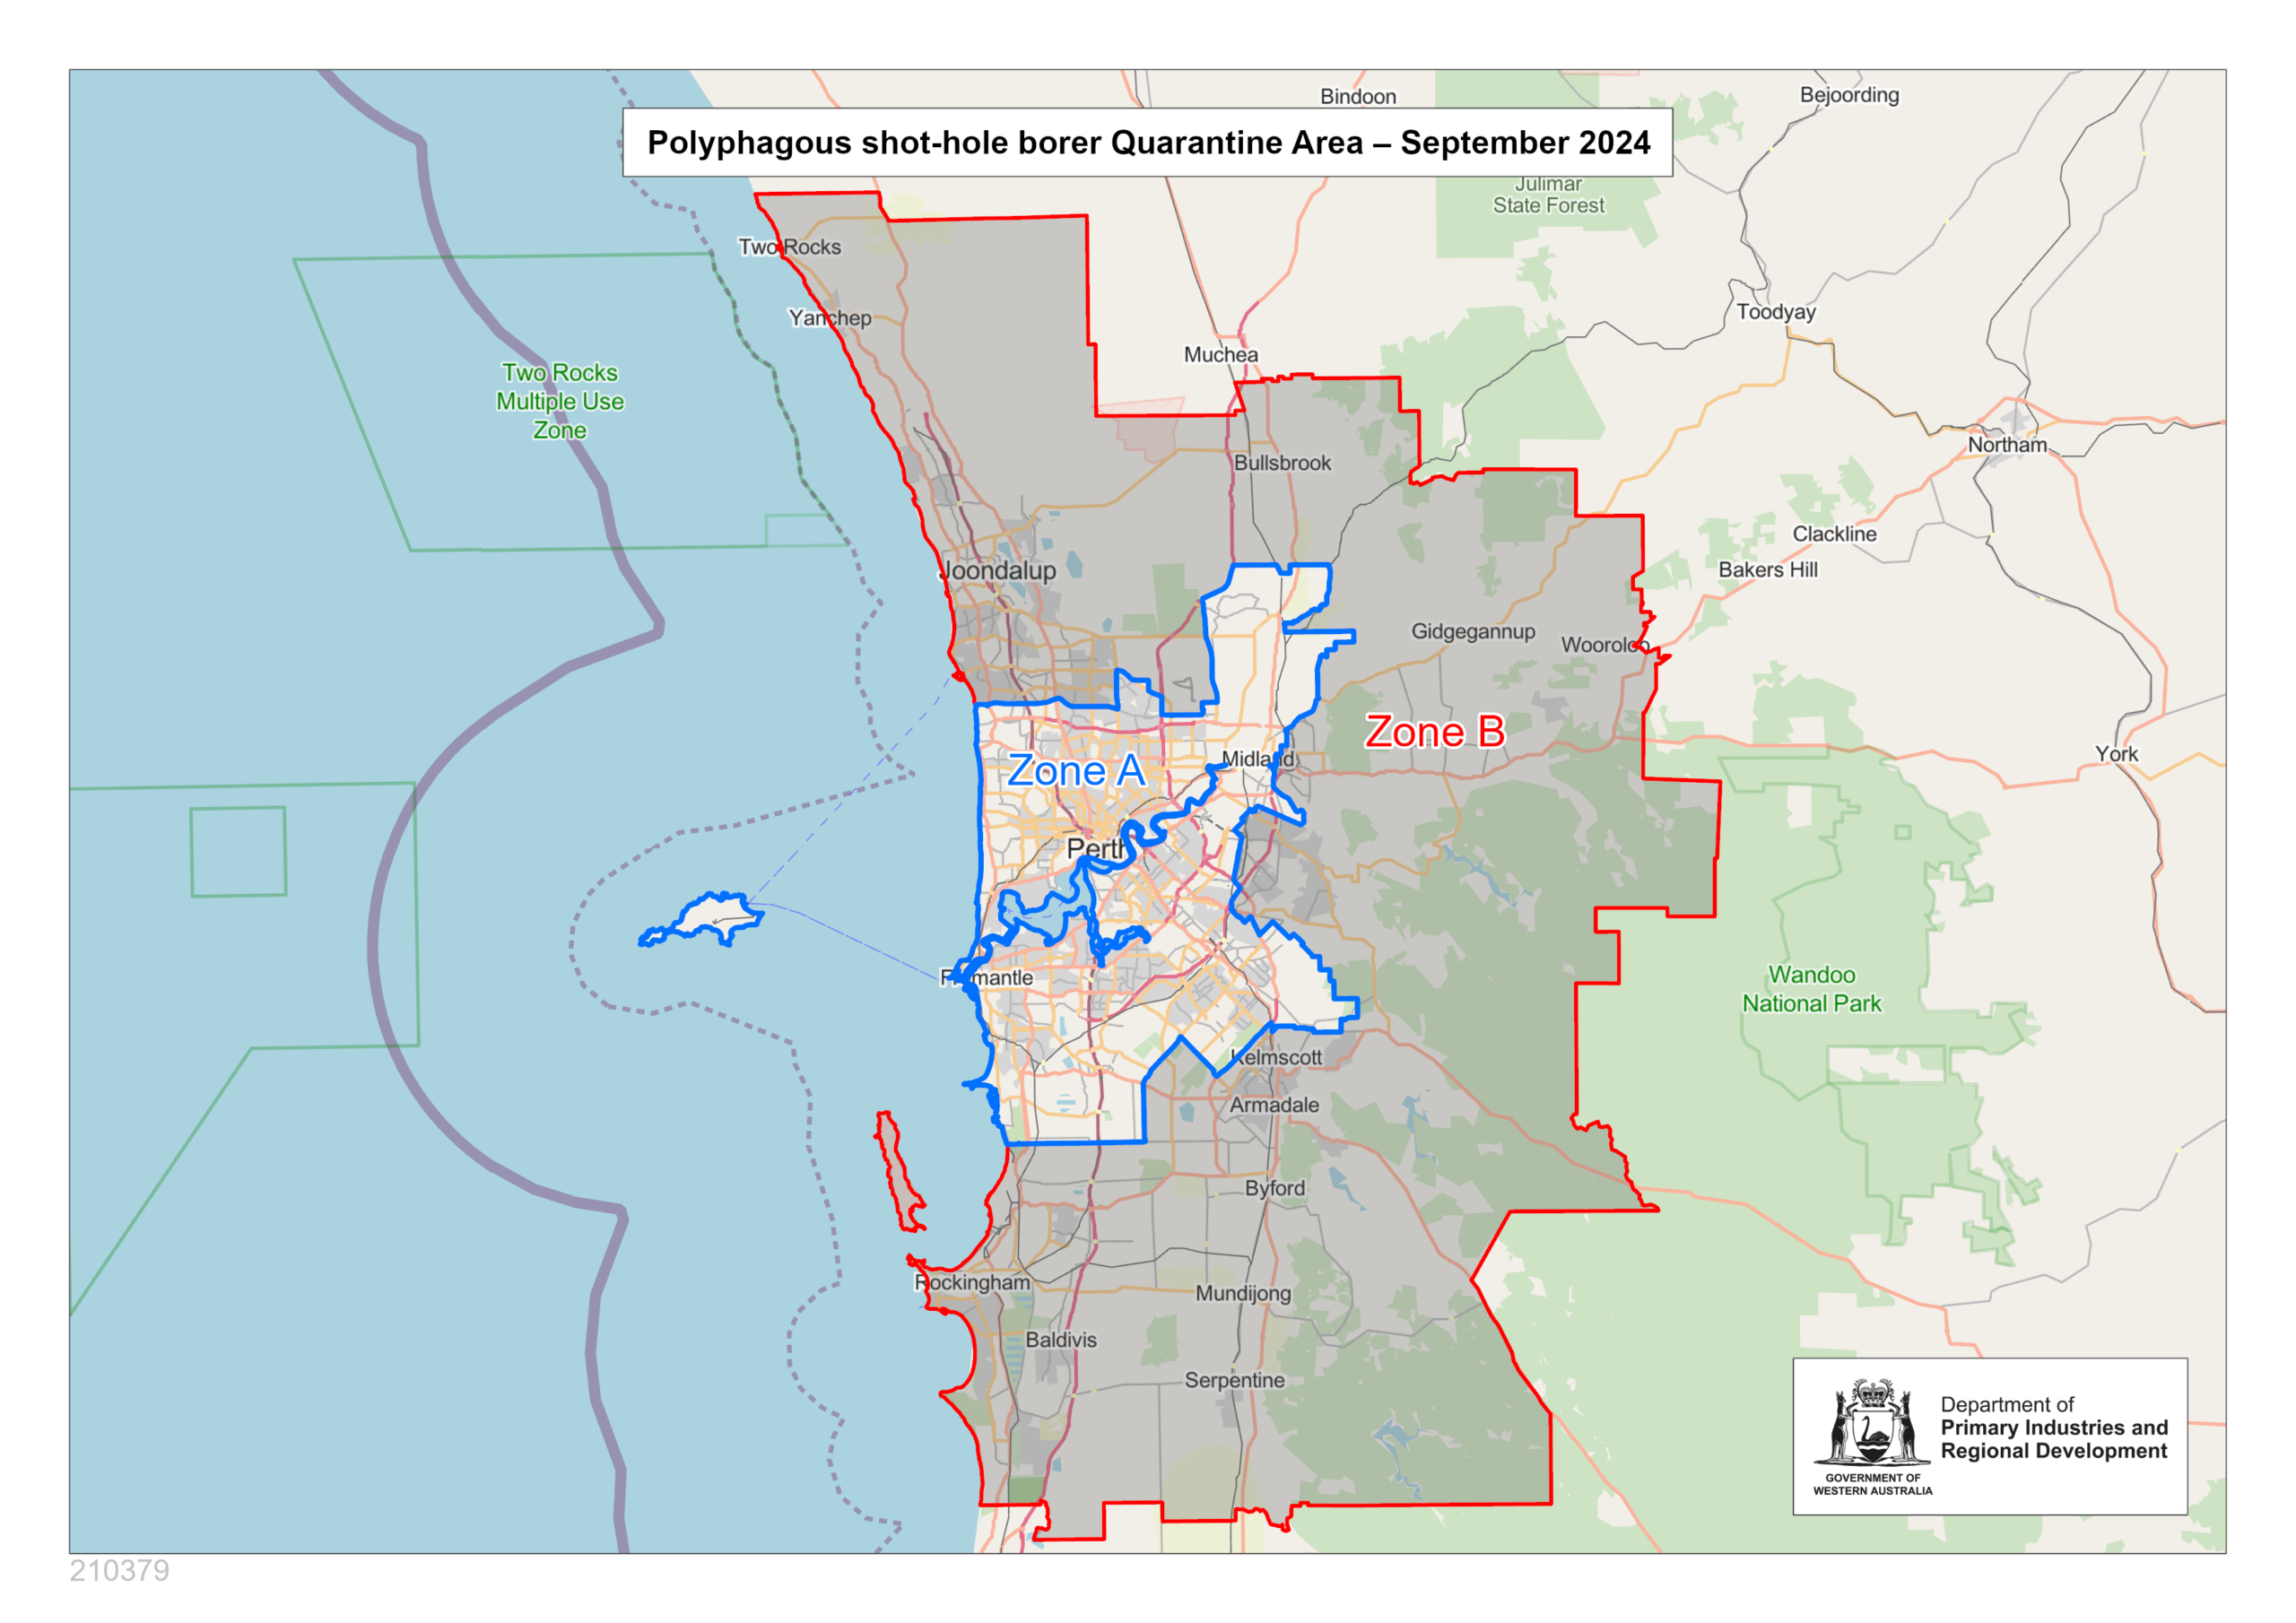
https://fadingforests.org

Floral richness of South Africa

Cape Coast lily (Crinum macowanii); photo by Jaqui Geux

South Africa is rich in plant diversity. That diversity is strongly shaped by the country’s varied topography, soils, & climate. Nine biomes & 465 vegetation types are recognized in a country of just 1.2 million km2 (471,445 square miles).

There is a long history of botanizing in southern Africa – with impressive results that include a Flora of the Southern Africa region (it covers Botswana, Eswatini, Lesotho, Namibia, as well as South Africa) and the African Plant Checklist & Database Project, which is the first continental checklist for Africa. This publication – which is being maintained continuously – contributes to goals of the Convention on Biological Diversity’s Global Strategy for Plant Conservation.

South Africans have also produced a national plant checklist that is updated every year. The most recent Checklist dates from 2025. The checklist includes bryophytes (mosses, hornworts, & liverworts), lycophytes & pteridophytes, gymnosperms, & angiosperms. Compilers plan to include marine macro-algae in future.

The 2025 checklist names 21,539 species in South Africa – 20,204 indigenous species, 1,329 naturalised species. Based on the, South Africa’s national flora comprises 5.3 % of the estimated ~ 380,000 plant species on Earth.

Geissoloma marginatum; photo by Tony Rebelo via Wikimedia

South Africa is home to 384 plant families, of which all but 34 contain only indigenous species. All the species in seven families are endemic to South Africa. These families are Bruniaceae, Geissolomataceae, Grubbiaceae, Lanariaceae, Penaeaceae (excl. Oliniaceae), Rhynchocalycaceae, & Roridulaceae. Of the 2,654 genera, 2,189 are indigenous. Three hundred (12%) of these genera are endemic. Sixty percent of the 20,204 indigenous species are endemic. All the endemic families other than Bruniaceae are composed of a single genus – demonstrating the phylogenetic uniqueness of this flora.

The 2025 Checklist contains 1,048 species that did not appear in the previous checklist (published in 2006). This is an increase of 4.9%. Numbers of indigenous taxa increased by less than 5%: additional 623 indigenous species (3.1%); 520 endemic species (4.3%). Numbers of non-indigenous species increased by considerably higher proportions: naturalized species increased by 414 species (31.1%), & invasive species by 451 (69.5%). These 865 species constitute 82.5% of all 1,048 newly recorded species. (I report the findings on non-indigenous species in a separate blog.)

The detection of previously unidentified species and infraspecific taxa – both native and non-indigenous – is the result of systemic botanizing campaigns focused on particular families. Thus, a study of the family Iridaceae in southern Africa led to description of 169 species in 20 genera. More than two decades of work on the Pelargonium (Geraniaceae) resulted in recognition of 34 new taxa. Thirty-three new species have been described in the genus Indigofera (Fabaceae).

The most specious plant family indigenous to South Africa is Asteraceae, with 2,124 species. Aizoaceae & Fabaceae follow with 1,603 & 1,566 species, respectively. The newly expanded Iridaceae is fourth; it encompasses 1,189 species. The world-famous Proteaceae rank 13th, with only 355 species. Considering genera, the largest by far is Erica (heath) at 734 species; no other genus houses more than 300 species. [The famous orchid genus Disa ranks 18th. There are ~182 species on the continent, primarily in East & Southern Africa.]

Disa uniflora on Table Mountain; F.T. Campbell

When considering phylogenies with high levels of endemism, the leading families are – again — Aizoaceae (1,426) and Asteraceae (1,352). Ranked third is Iridaceae (983). Fabaceae is ranked 4th (961). Nearly half (49%) of species in 1,071 genera are endemic. Again Erica ranks highest: 581 species – 78% of the species in the genus – are endemic. This is double the number in the genus ranked second — Aspalanthus (261species; all but 34 species are endemic). Pelargonium is 3rd : 204 of 261 species are endemic.

Flora of the provinces

 Of South Africa’s nine provinces, KwaZulu-Natal (94,361 km2) is home to the greatest diversity in terms of plant families (331 families) and genera (1,718 genera). Neighboring Eastern Cape Province (168,966 km2) ranks second with 305 families and 1,576 genera. Western Cape has somewhat fewer plant families (294) and genera (1,475), but by far the most species (11,379). Western Cape also leads in the proportion of its plant taxa that are endemic to the province: 58%. (This reflects the presence of a globally recognized distinct flora, the Cape Floral Kingdom.) KwaZulu-Natal and Eastern Cape (16% endemic) share most of their plant taxa with neighboring provinces or countries – Mozambique. Therefore, their levels of endemism are only 8% and 16%, respectively.

The clustering plant diversity and endemism in the south & east reflects the topographic variation provided by the Escarpment of South Africa.

The largest province is Northern Cape Province at 372,889 km2. It is home to 5,058 species but its fairly uniform terrain means there is not very high species diversity (25 % – half the proportion in Western Cape). However, the flora is unique because adapted to the harsh environment (I concede these statements seem contradictory).

Pachypodium namaquanam; F.T. Campbell

SOURCE

Le Roux, M.M., R.R. Klopper. 2025. Taking stock of South Africa’s flora. South African Journal of Botany 184 (2025) 571-579

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
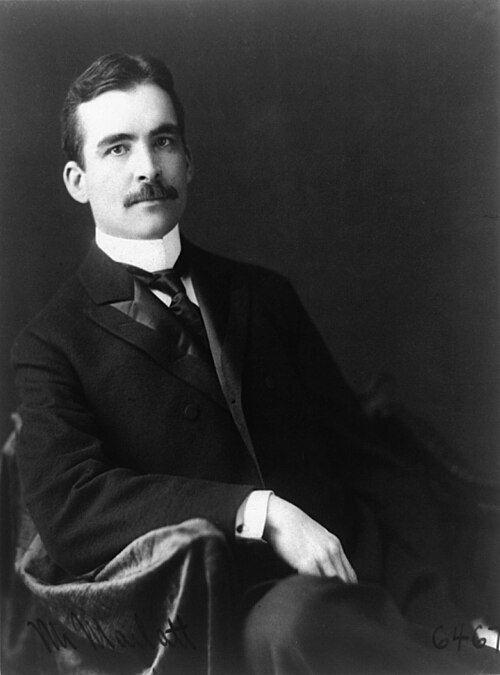
https://fadingforests.org

Factoids from recent publications

Agrilus auroguttatus

Agrilus genus

Hernández‐Gutiérrez, Nichols, and Kelly (2026) (full citation at the end of the blog) analyzed interactions between this genus of beetles and oaks (Quercus species). In this context, they report that 32 Agrilus species from Africa, Asia, Europe, and North and South America use 51 Quercus species as hosts in their native range. Eighteen (56.25%) use only Quercus hosts.

Oaks that host Agrilus species cluster in several clades, i.e., the entire Section Cerris and one clade of Section Ilex and two clades of section Lobatae. Clades where Agrilus hosts are underrepresented are Sections Cyclobalanopsis and Quercus &, surprisingly, two clades in Section Lobatae.  

Their analysis indicated that beetle-oak interactions involving all the 32 Agrilus species and 105 Quercus species in their study had a significant likelihood of being damaging. For example, northern red oak (Q. rubra) is already known to host six Agrilus species. Hernández‐Gutiérrez, Nichols, and Kelly (2026)’s analysis indicated that this tree species might be utilized by all 32 Agrilus species assessed. The tree’s wide distribution (both native and introduced) places it close to other known or probable hosts, which exacerbates the risk of an interaction. Another 26 Quercus species are predicted to host ten or more Agrilus species.

The model was not successful in predicting hosts of A. auroguttatus (goldspotted oakborer) in its introduced range in California.

black oak (Quercus kelloggii) in Cleveland National Forest killed by GSOB; photo by F.T. Campbell

It also predicted that few of China’s oak species might host Agrilus beetles. However, as Dr. Robert Haack notes (pers. comm. June 2026), larval hosts have been identified for only 13% of the nearly 1,200 Asian Agrilus.

Some Agrilus species have a very large number of predicted novel interactions. A. graminis and A. angustulus are predicted to have more than 40 novel oak hosts. Both have numerous known oak hosts; so their “polyphagous” nature is already documented.

Since two-thirds of 666 Agrilus species with known larval hosts exploit only one plant genus as a host in their native range, Hernández‐Gutiérrez, Nichols, and Kelly (2026) assert that they might spread faster if introduced to homogeneous rather than species-rich habitats. Dr. Haack believes that this statement is too broad (pers. comm. June 2026).

A. bilineatus; photo by Christina Butler via Wikimedia

Twolined chestnut borer

Haack and Blank (2024) document that the twolined chestnut borer, Agrilus bilineatus has preferentially infested apparently healthy English oak (Quercus robur) trees over healthy native oak trees in Michigan. In North America, A. bilineatus is a major pest of oaks and American chestnut (Castanea dentata)when they are stressed by drought or other factors. Infestation typically begins in the upper crown and proceeds downward; tree death often occurs within three years.

 At several sites in southern Michigan, where English oaks were intermixed with native white oaks (Quercus alba) and close to northern red oaks (Quercus rubra), A. bilineatus preferentially infested Q. robur trees that initially appeared healthy. Further study revealed that many of the English oaks attacked had low or depleted root starch levels.

Although these findings are cause for alarm, English oak is already used by 11 species of Agrilus in Europe. Perhaps the tree and ecosystem might have sufficient defenses in Europe. Meanwhile, A. bilineatus has been reported in Turkey as of 2018; I have found no recent information about the damage whether it is causing any damage there.

Data from Britain and Worldwide

Peyton et al. (2026) reviewed the effectiveness of a “horizon scanning” exercise conducted for Great Britain (England, Scotland and Wales). They report that 3,248 recognized non-native species have been detected in Great Britain, of which 2,016 have established self-sustaining populations. Some 194 (~10%) are considered invasive, that is, have negative impacts on biodiversity and wider ecosystem viability. These consist of 108 terrestrial species, 47 freshwater species, and 39 marine species. These bioinvaders cost the British economy an estimated ~£3.9 billion per year (the bulk of the damage is attributed to ash dieback, caused by the fungus Hymenoscyphus fraxineus).

In the decade between completion of the “horizon scan” and the present, 143 species were recorded as being introduced. The horizon scan predicted 31 of these species, 22%. Peyton et al. (2026) consider this to be success.

Peyton et al. (2026) report that globally, ~ 6% of non-native plant species are ranked as invasive. Among invertebrates, this proportion rises to 22%. Considering vertebrates introduced to Europe or North America, the figure is more than 50%!! I welcome global data that support my call for rethinking the “rule of tens” long relied on for estimating the proportion of non-native species that are invasive.  

Discussing bioinvaders’ role in causing extinctions, Peyton et al. (2026) report that 30 predators have been linked to declines and extinctions of 738 vertebrate species.

Peyton et al. (2026) also discuss the difficulty in predicting an introduced species’ impacts when in some cases the time lag between introduction and presence in the wild or between establishment and spread w/in the region can last decades or even a century. They cite as an example Senecio squalidus, which escaped the Oxford Botanic Gardens in the 1700s but started to spread only during mid-1900s.

Australia

More than 300 non-native insect pests, pathogens and nematodes have established on tree or shrub hosts in Australia; 20% have caused moderate to high impacts to commercial plantations, urban forests, or trees in natural ecosystems (Carnegie et al. 2026).The rate at which non-native forest pests and pathogens have been detected in Australia has doubled since 2018 compared to earlier decades: from ~ 1.5 to ~ 3 per year. Carnegie et al. (2026) attribute this rise to greatly expanded official surveillance efforts. Still, three-quarters of the most recent detections came too late for eradication to be attempted.

The Forestwatch program (inaugurated – under a different name – in 2022) includes pathogens. I rejoice!!! Still, the target species threaten primarily tree species not native to Australia but important to commercial forestry or urban forests: Asian longhorned beetle,  burnt pine longicorn (Arhopalus ferus), pine pitch canker, pine wilt disease, red turpentine beetle (Dendroctonus valens), Asian spongy moth, red needle cast, and sudden oak death. The exceptions are strains of Austropuccinia psidii not yet intro to Australia, and eucalypt leaf blight (caused by Teratosphaeria destructans) (Carnegie et al. 2026).

Austropuccinia psidii infection on Melaleuca in Australia; photo by John Tann via Flickr

Among the introduced pests causing the greatest damage to native species are

  • Phytophthora cinnamomi: this soil fungus can kill 40% of the plant species in the southern portion of Western Australia  – which is one of 36 “Biodiversity Hotspots” recognized by the Critical Ecosystem Partnership Fund.  
  • Austropuccinia psidii (cause of myrtle rust) in natural ecosystems; Members of the host family Myrtaceae occur in 11 of 13 major vegetation formations on Australia. Various authorities have identified 76 species as at risk to the rust.

I hope the Australians are developing strategies for landowners to counter damage by the polyphagous shot hole borer (Euwallacea fornicatus) and its associated fungus (Fusarium euwallaceae). DMF Outbreak detected near Perth, Western Australia, in 2021 – apparently three years after the actual introduction. By June 2025 authorities had determined that it was too widespread to be eradicated, so landowners will be responsible for any management.  (Carnegie et al. 2026) Impact is predicted to be greatest in urban landscapes, and cost up to AU$9.7 M per annum to manage.

Phytophthora pluvivora was first detected in Australia on an English oak, Quercus robur. However, it has since been recorded on native species in the Blue Mountains, including the critically endangered dwarf mountain pine (Pherosphaera fitzgeraldii) in a National Park.

SOURCES

Carnegie. A.J., B.A. Summerell, C. Trollip, F. Tovar, D.I. Smith, and J. McDonald. 2026. Sentinel trees for early detection of non-native forest pests and pathogens in Australia. Front. For. Glob. Change 9:1801183. doi: 10.3389/ffgc.2026.1801183

Haack, R.A. and R.B. Blank. 2025.  Susceptibility of English Oak (Quercus robur) to the Twolined Chestnut Borer, Agrilus bilineatus (Coleoptera: Buprestidae): Observations from Michigan. The Great Lakes Entomologist. 57: 113-125. https://doi.org/10.22543/0090-0222.2492

Hernández‐Gutiérrez, E., R.A. Nichols, and L.J. Kelly. 2026. Combined phylogenetic and geographic data can predict plant–pest interactions with high accuracy. New Phytologist (2026) doi: 10.1111/nph.71306

Peyton, J.M., S. Rorke, D.C. Aldridge, O.L. Pescott, K. Dehnen- Schmutz, D.G. Noble,  J. Sewell, A.J.A. Stewart,  T. Adriaens,  B.C. Beckmann,  J. R. Britton, J. Brodie1, P.M.J. Brown, I.C.N. Cavadino, P.F. Clark, A.M. Dunn, J.Foster, C. Harrower, M.C. Harvey, M.C. Jackson, T. Jones, C.A. Maggs, G. Martin, F. Mathews, A.C. Mill, D. Murphy,  E. Paganini, R. Payne, W. Rabitsch, T. Renals,    K. Schönrogge, R.H. Shaw, G.C. Smith, P.D. Stebbing, P.A. Stroh, H. Tidbury, E. Tricarico, J. Vallet,   K.J. Walker, L.E. Wood, C.A. Wood, B. Woodcock, H.E. Roy. 2026. Assessing the success of a horizon scanning approach in predicting invasive non- native species arrival. J Appl Ecol. 2026;63: https://doi.org/10.1111/1365-2664.70217

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
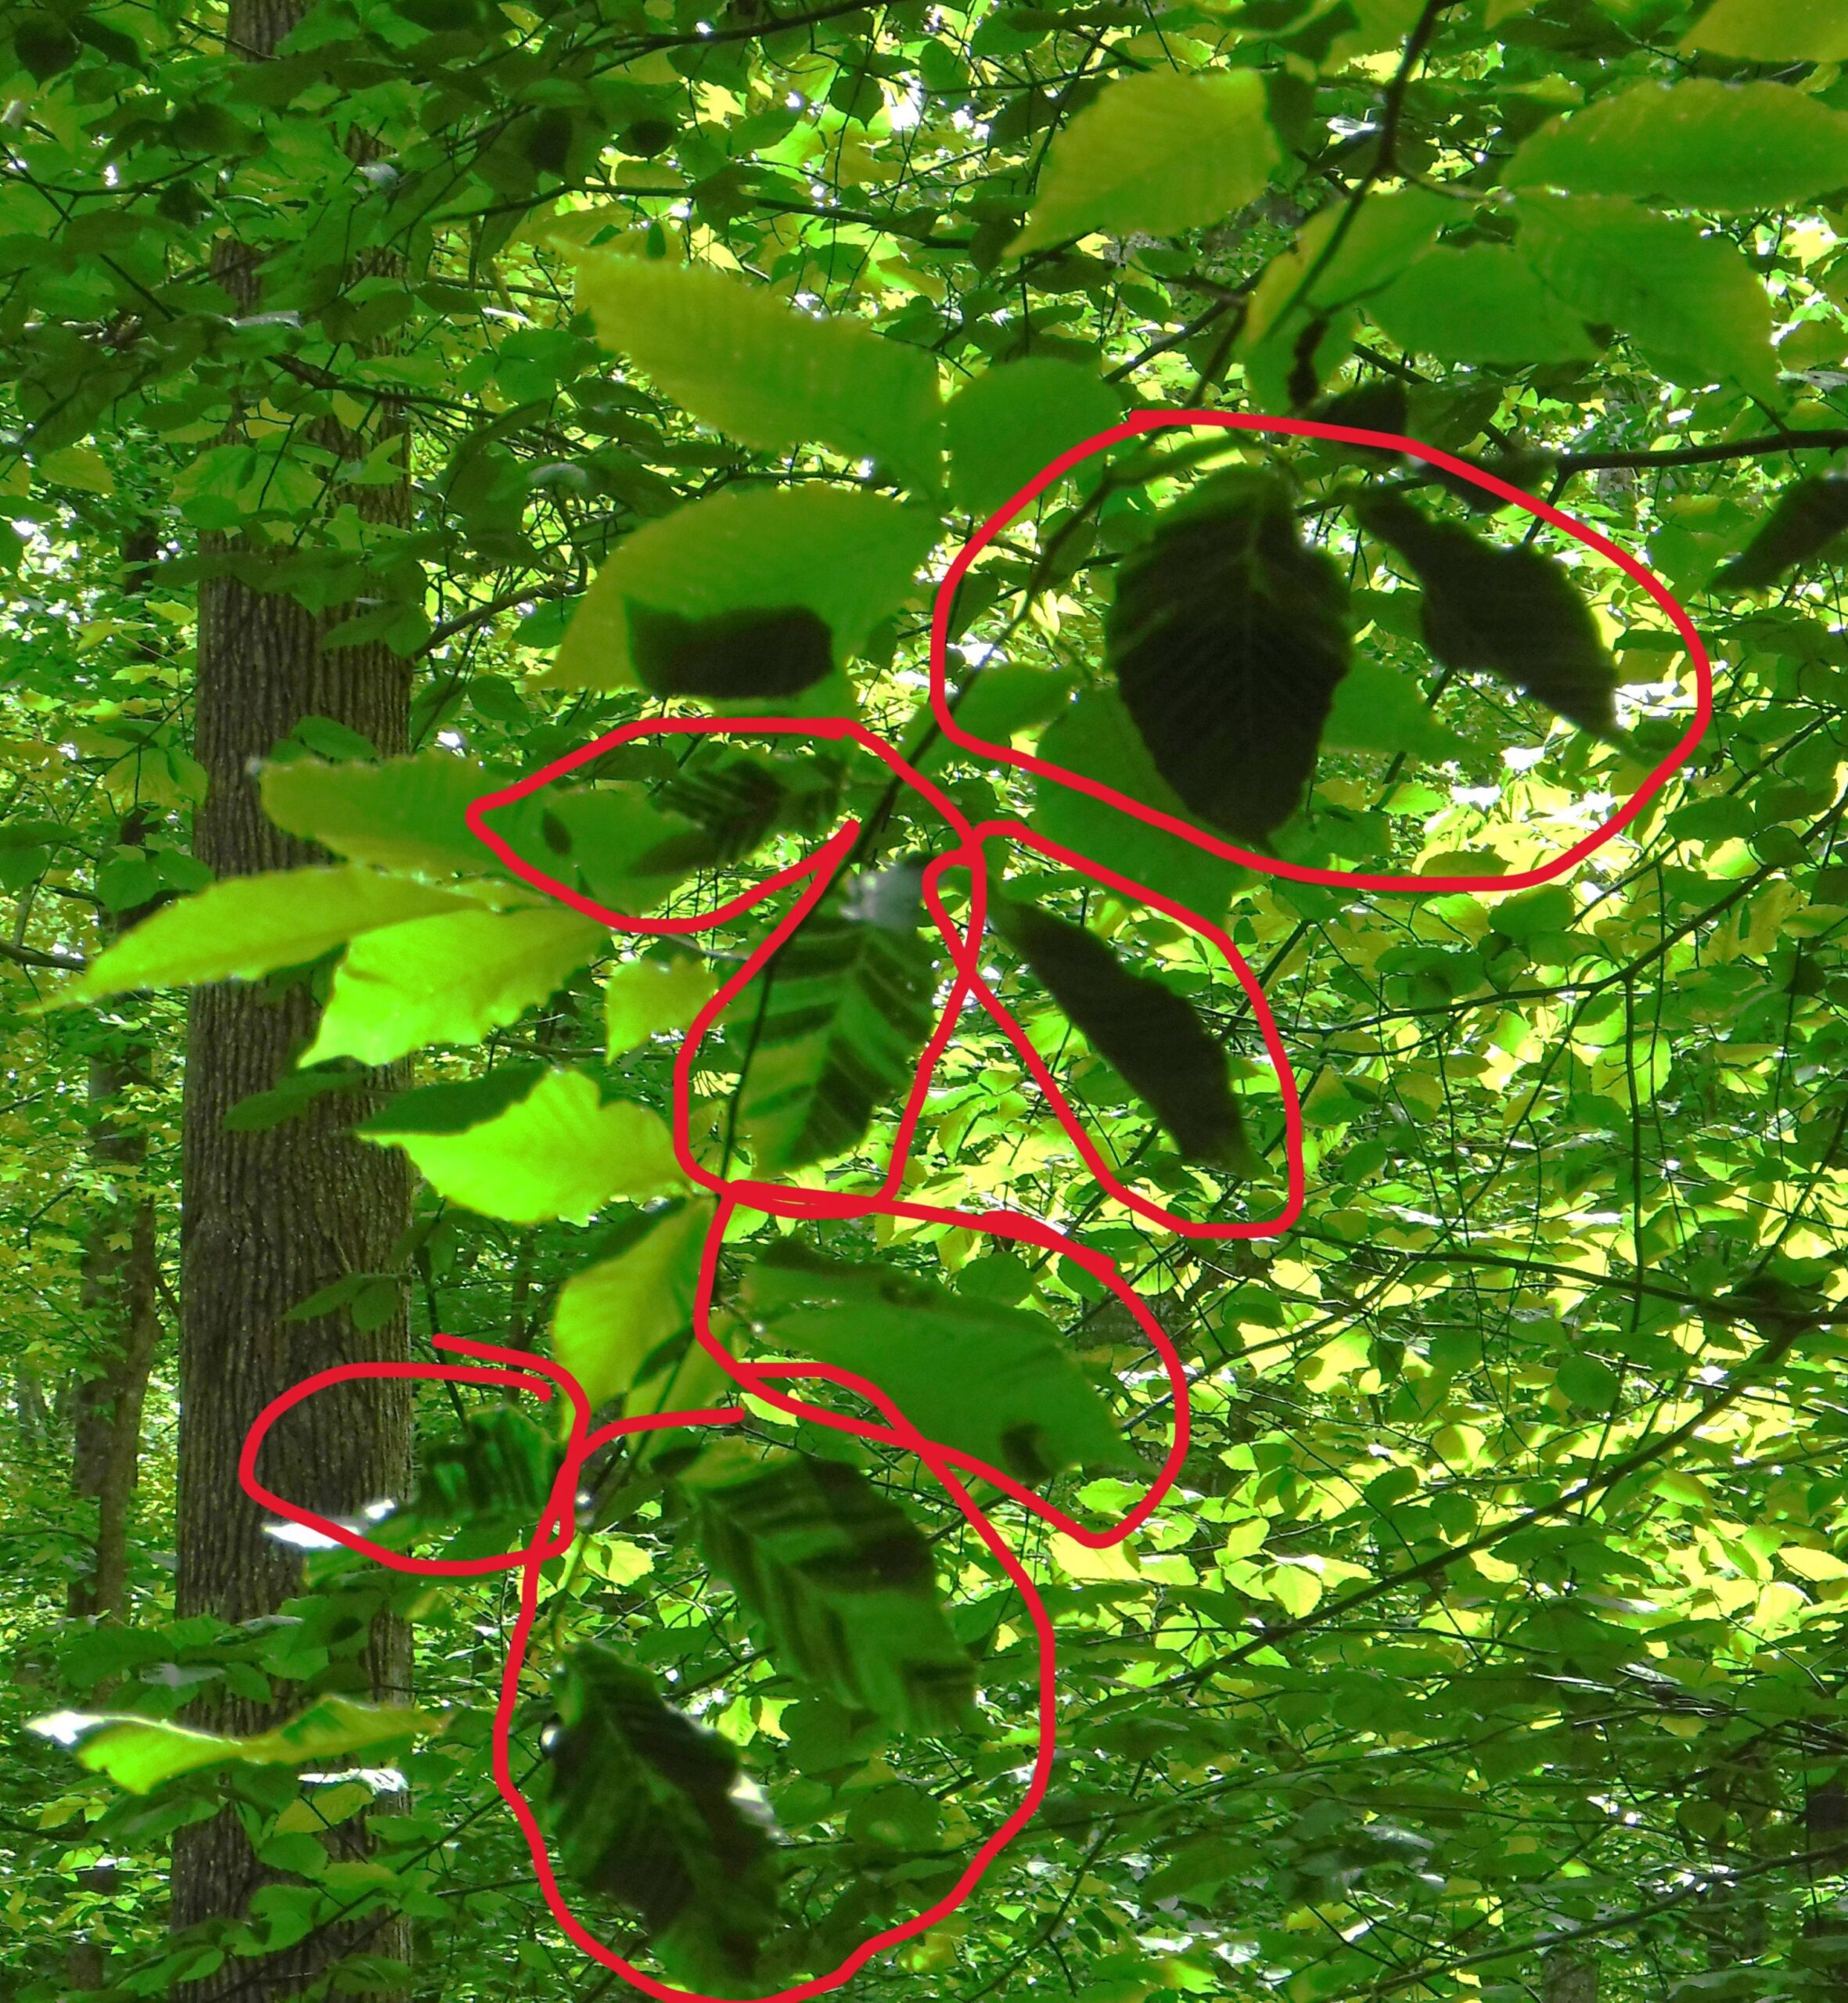
https://fadingforests.org