The invasive risk of Eucalypts

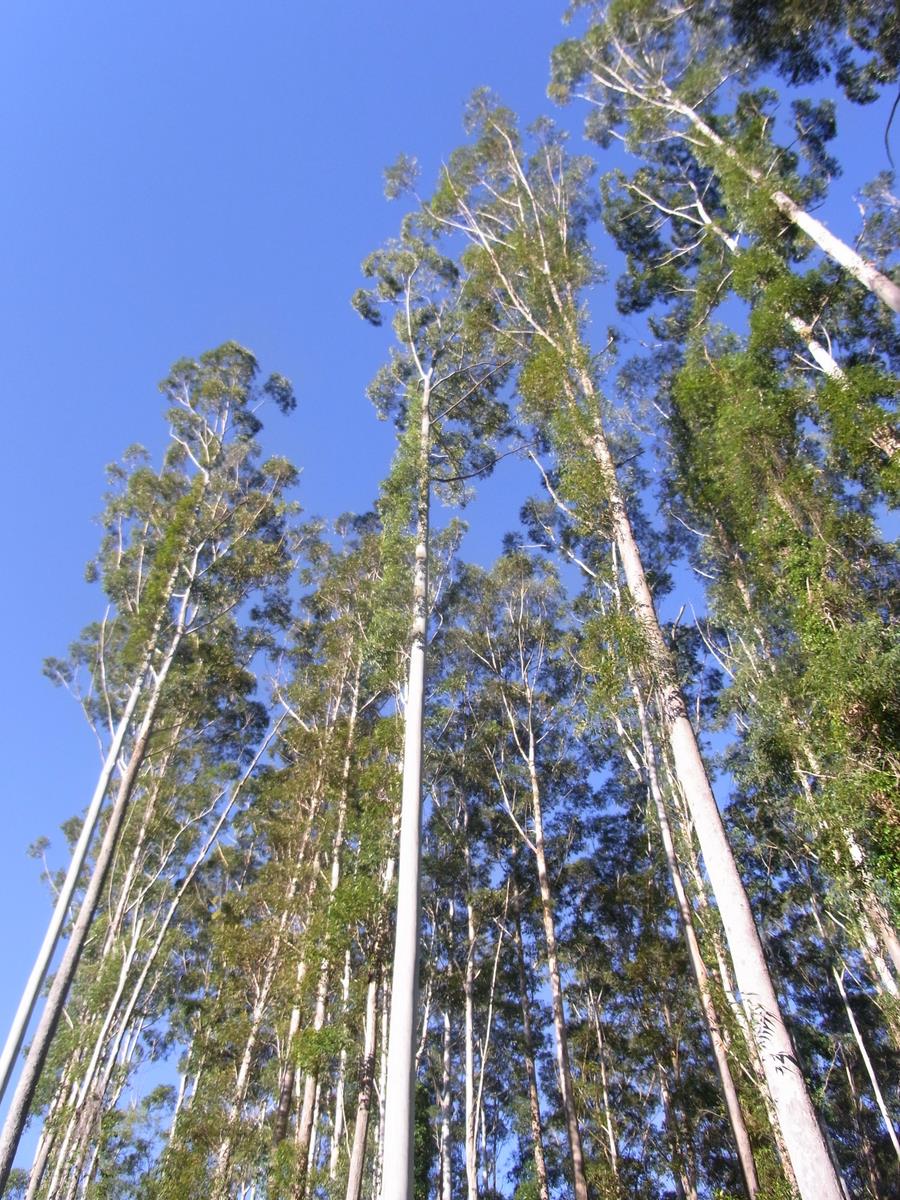
Eucalyptus grandis (in Australia); photo by Poyt448 Peter Woodard via Wikimedia

Deus et al. 2025 (full citation at the end of this blog) have published a review of current knowledge on the invasiveness of trees in the Eucalyptus genus. They report that eucalypt plantations cover more than 30 million ha globally; they could not determine the actual extent more precisely. The area is expanding at an estimated 4% per year. Eucalypts are so popular as timber trees because of their fast growth, ease of management, wood quality and environmental tolerance.

Until recently, trees in the Eucalyptus genus were thought to pose a low invasion risk. This was because these trees have limited seed dispersal, high juvenile mortality, and were expected to lack compatible ectomycorrhizal fungi in novel environments. However, several risk assessments and reports of ongoing invasions in some locations have raised questions. So Deus et al. undertook a literature survey to try to resolve the issue.

One of the risk assessments concerns the United States; see Gordon et al. (2012). This study – completed a dozen years before Deus et al. undertook their literature survey – cited several other sources documenting harmful invasiveness of nearly a dozen species, including Eucalyptus globulus, E. camaldulensis, E. grandis, and  E. tereticornis.

Deus et al. found that the limitations listed above actually can be overcome, so they do not prevent invasions:

  • seeds can disperse farther than 100 meters from parent plants;
  • high recruitment densities can compensate for the high juvenile mortality; and
  • ectomychorrhizal fungi can be found in the root systems of introduced eucalypt plants.

In fact, several Eucalyptus species meet criteria defining invasiveness in the Australian Weed Risk Assessment system. Still, Deus et al. found that existing studies cover too few plantations and species to allow an in-depth comprehensive understanding of eucalypts’ invasion ecology.

One reason that eucalypt trees’ invasiveness remains unresolved is that the countries which have established most large Eucalyptus plantations (Brazil, India and China) have not conducted many studies. Instead, most studies have been done in Iberia and South Africa, which together host less than six percent by area of the world’s estate of eucalypt plantations.

Deus et al. say that several possible reasons have been proposed to explain why Eucalyptus is considered to pose an invasion risk by scientists in Iberia and South Africa, but not in Brazil. 

  1. The few studies in Brazil were conducted in intensively managed plantations with very short rotations, which are probably less prone to invasion than plantations managed at low intensity levels.
  2. The Brazilian plantations were established 40 to 50 years ago, whereas those in Iberia were introduced ~ 200 years ago.
  3. Iberia experiences recurrent forest fires.
  4. In Brazil, leaf eating ants attack the trees; this might reduce trees’ vigor.
  5. In Brazil, native forests dominate the environs.

Deus et al. say that these hypotheses have never been tested.

Since studies have been conducted in only a few countries, they have evaluated only a few of the species used in plantations. At least 372eucalypt species have been introduced outside their native range; nine species are planted widely. Yet most of the studies reviewed by Deus et al. covered just two species, Eucalyptus globulus (46% of the studies), and E. camaldulensis (33% of the studies). Still, these two widely cultivated species received the highest invasiveness ranking of all species reviewed (65 and 72, respectively). According to Deus et al., these scores are higher than the average score for 32 species of Acacia – a genus considered to be one of the most invasive tree genera in the world.

Other, potentially invasive species, have not received adequate attention. Deus et al. note that E. tereticornis, which is widely planted in China, India and other regions of Southern Asia, has an invasiveness score of 66, placing it second highest in the evaluation. However, only 12 of 140 articles analyzed by Deus et al. addressed this species.

These eucalypts’ high scores result from their potential to hybridize, to naturalize outside their natural habitat, and from high flammability. Other contributing factors are high seed production and ability to resprout after cutting or fire.

The analysis determined that the major drivers for Eucalyptus invasions are soil disturbance, availability of moisture (essential for seedling establishment), and fire. Recruitment density increases with harvesting and tree age; it decreases when the understory is managed. This partially explains why the abandonment of plantations might promote invasions by eucalypts.

Deus et al. fear that there might be a large “invasion debt” in the regions where few studies have been conducted. Assessments for California and Iberian Peninsula indicate that the best areas for cultivation – under either current conditions or expected new environments linked to climate change – are also those most prone to invasion. A further complication is that in some regions it might be difficult to distinguish plants escaping from small plantations from the plantations themselves. They suggest ways to overcome this difficulty: 1) surveys of recruitment along roadside, where trees would not have been planted; 2) genetic analysis of seedlings and possible parents

Another weakness is that that none of the studies considers changes in fire regime, which probably increases the areas prone to invasion.

Deus et al. think it is unlikely that eucalypt invasions will turn out to be as damaging as those of acacias or pines, but that further invasions involving more species and more regions are very likely.

Deus et al. call for considering eucalypt species’ potential invasiveness when developing strategies for the sustainable management of these plantations, including how to manage those that are no longer economically viable.

Status in the United States

The risk in the United States was evaluated by Gordon et al. in 2012. At the time, there were proposals to plant 5,000 to 10,000 ha/year in the Southeast over the next decade.
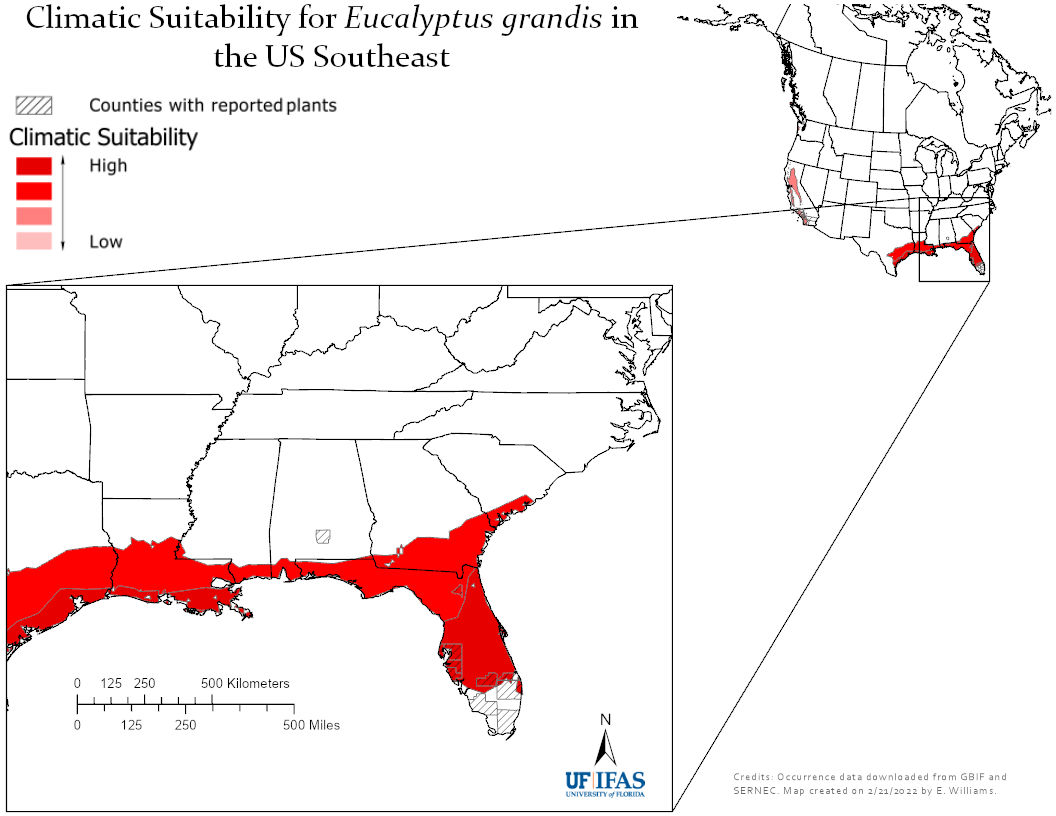
Gordon et al. adapted the Australian weed risk assessment system to evaluate 38 Eucalyptus taxa then being tested and cultivated in U.S. for pulp, biofuel, and other purposes. Their analysis concluded that 15 of these taxa posed a low risk; 14 taxa posed a high risk; and 9 taxa could not be ranked without further information. The four taxa cultivated most extensively –  E. globulus, E. camaldulensis, E. grandis, and E. tereticornis – all had high risk outcomes, as did several other taxa. Gordon et al. thought that these differences reflected both new data and differences in how the assessors reacted to insufficient data.

Gordon et al. warned that novel genotypes with unknown invasiveness were being propagated in the search for increased cold tolerance. This meant that the taxa they had assessed might not indicate of the actual long-term invasion risks associated from this genus. A major source of uncertainty is the long lag time in appearance of evidence of a tree species’ invasiveness. Only one study (as of 2012) had quantified lag time for introduced tree species; it found an average of 170 years from the time introduction to identification of the taxon as invasive. Propagule pressure also influences the lag time and the probability of invasion.

Since the bulk of expanded cultivation was expected to be in the southeast, Gordon et al. recommended that a regional assessment be conducted to more precisely specify the effects of possible differences in phenology, age at reproductive maturity, seed viability, and cold tolerance. 

Gordon et al. suggested several actions to reduce the invasion risk. First, selection and breeding strategies could aim to minimize relevant traits – especially eliminating seed production. Second, plantations could be so managed by avoiding cultivation near waterways, harvesting stems before seeds can mature, and restricting the extent of cultivation of any one taxon. More broadly, a fund could be established to cover control costs; growers would contribute the money.

What has happened in the dozen years since the analysis was published? My Google search led to publications from 2013 and earlier. I hope this indicates that no one has funded major expansions. Dr. Gordon reports that most Eucalyptus pulp is imported. ArborGen continues to breed Eucalyptus in Brazil – as I noted earlier, scientists there are not pursuing studies of possible invasiveness of eucalypts.

Still, the regional risk assessment has not been conducted. Worse, Dr. Gordon reports that the Florida Department of Agriculture and Consumer Services has exempted several species [E. amplifolia, E. benthamii, E. dorrigoensis, E. dunnii, E. grandis, E. gunni, E. nitens, E. smithii, and E. urograndis (E. grandis  E. urophylla)] from a requirement that growers obtain Non-Native Species Planting Permits. So if the market does take off, there will be no regulation by the state.

At the end of December 2025, Dr. Gordon received information from Florida Division of Plant Industry that no one has applied for a permit to grow Eucalyptus in the state other than under USDA research auspices. So my worst fears have not (yet) come to pass.

I note that in 2022, Potter, Riitters, & Guo ranked Eucalyptus grandis & E. globulus as potentially highly invasive. Their criterion was that at least 75% of stems detected by USFS Forest Inventory and Analysis (FIA) surveys were saplings or seedlings.

SOURCES

Deus, E., D.M. Richardson, F.X. Catry, F.C. Rego, J. Gaspar, M. Nereu, M. Larcombe, B. Potts, J.S. Silva. 2025. Invasion ecology of eucalypts: a review. Biol. Invasions (2025) 27:239  https://doi.org/10/1007/s10530-025-03695-1

Gordon, D.R.,S.L. Flory,.L. Cooper, and S.K. Morris. 2012. Assessing the Invasion Risk of Eucalyptus in the United States Using the Australian Weed Risk Assessment. International Journal of Forestry Research Volume 2012, Article ID 203768, 7 pages doi:10.1155/2012/203768

Potter K.M., Riitters, K.H. & Guo, Q. 2022. NIS tree regeneration indicates regional & national risks from current invasions. Frontiers in Forests & Global Change  

doi: 10.3389/ffgc.2022.966407

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Welcome high-level attention to bioinvasions – although key issues remain unresolved

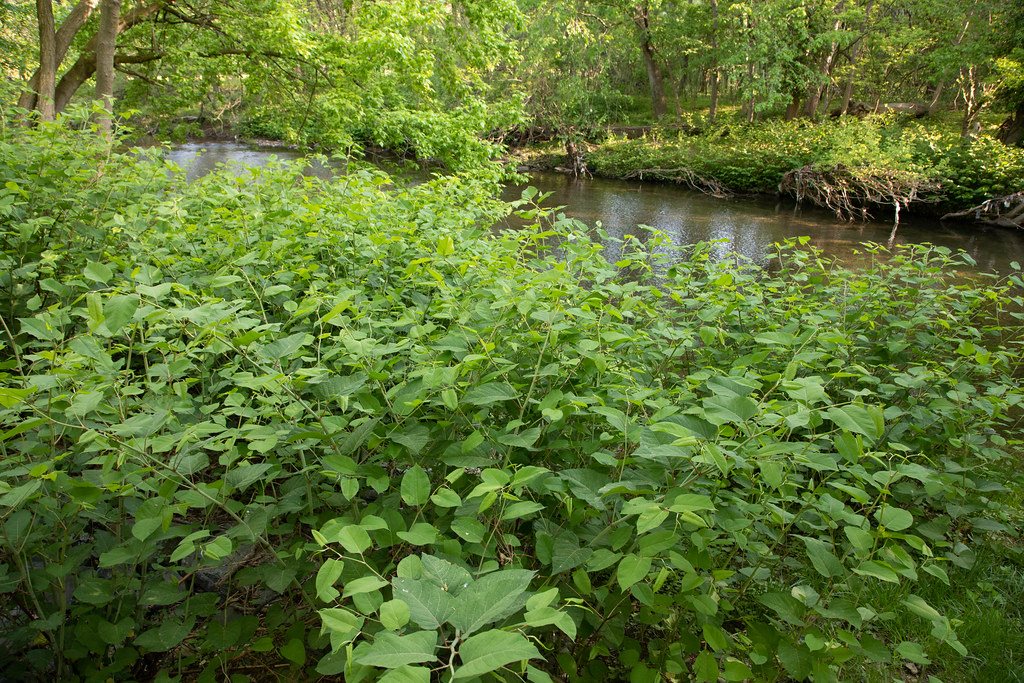
Japanese knotweed (Reynoutria japonica) – one of the worst invaders around globe. Photo by Will Parson, Chesapeake Bay Program via Flickr

On 23 October, Science published a five-page, data-packed analysis of bioinvasion impacts on terrestrial ecosystems!!! 

Thakur, Gu, van Kleunen, and Zhou (full citation at end of this blog) analyzed 775 studies with the goal of improving understanding of factors contributing to invasions’ impacts – as distinct from “invasibility” (ability to establish). This knowledge is essential to assessing the risk posed by introduced species and setting priorities for management. They analyzed five ecological contexts—diversity of native species and introduced species in the recipient systems, latitude, invader residence time, and invader traits.

They concluded that ecological factors commonly used to explain invasion success do not consistently translate into strong predictors of invasion impacts. Impacts vary in response to the context of the invasion.

[In January 2026, the authors announced changes in details of the article due to some errors in the database and their understanding of it. (Science 8 Jan 2026 Vol. 391 Issue 6781) They conclude that the corrected analysis did not alter the trends described or the overall conclusions.]

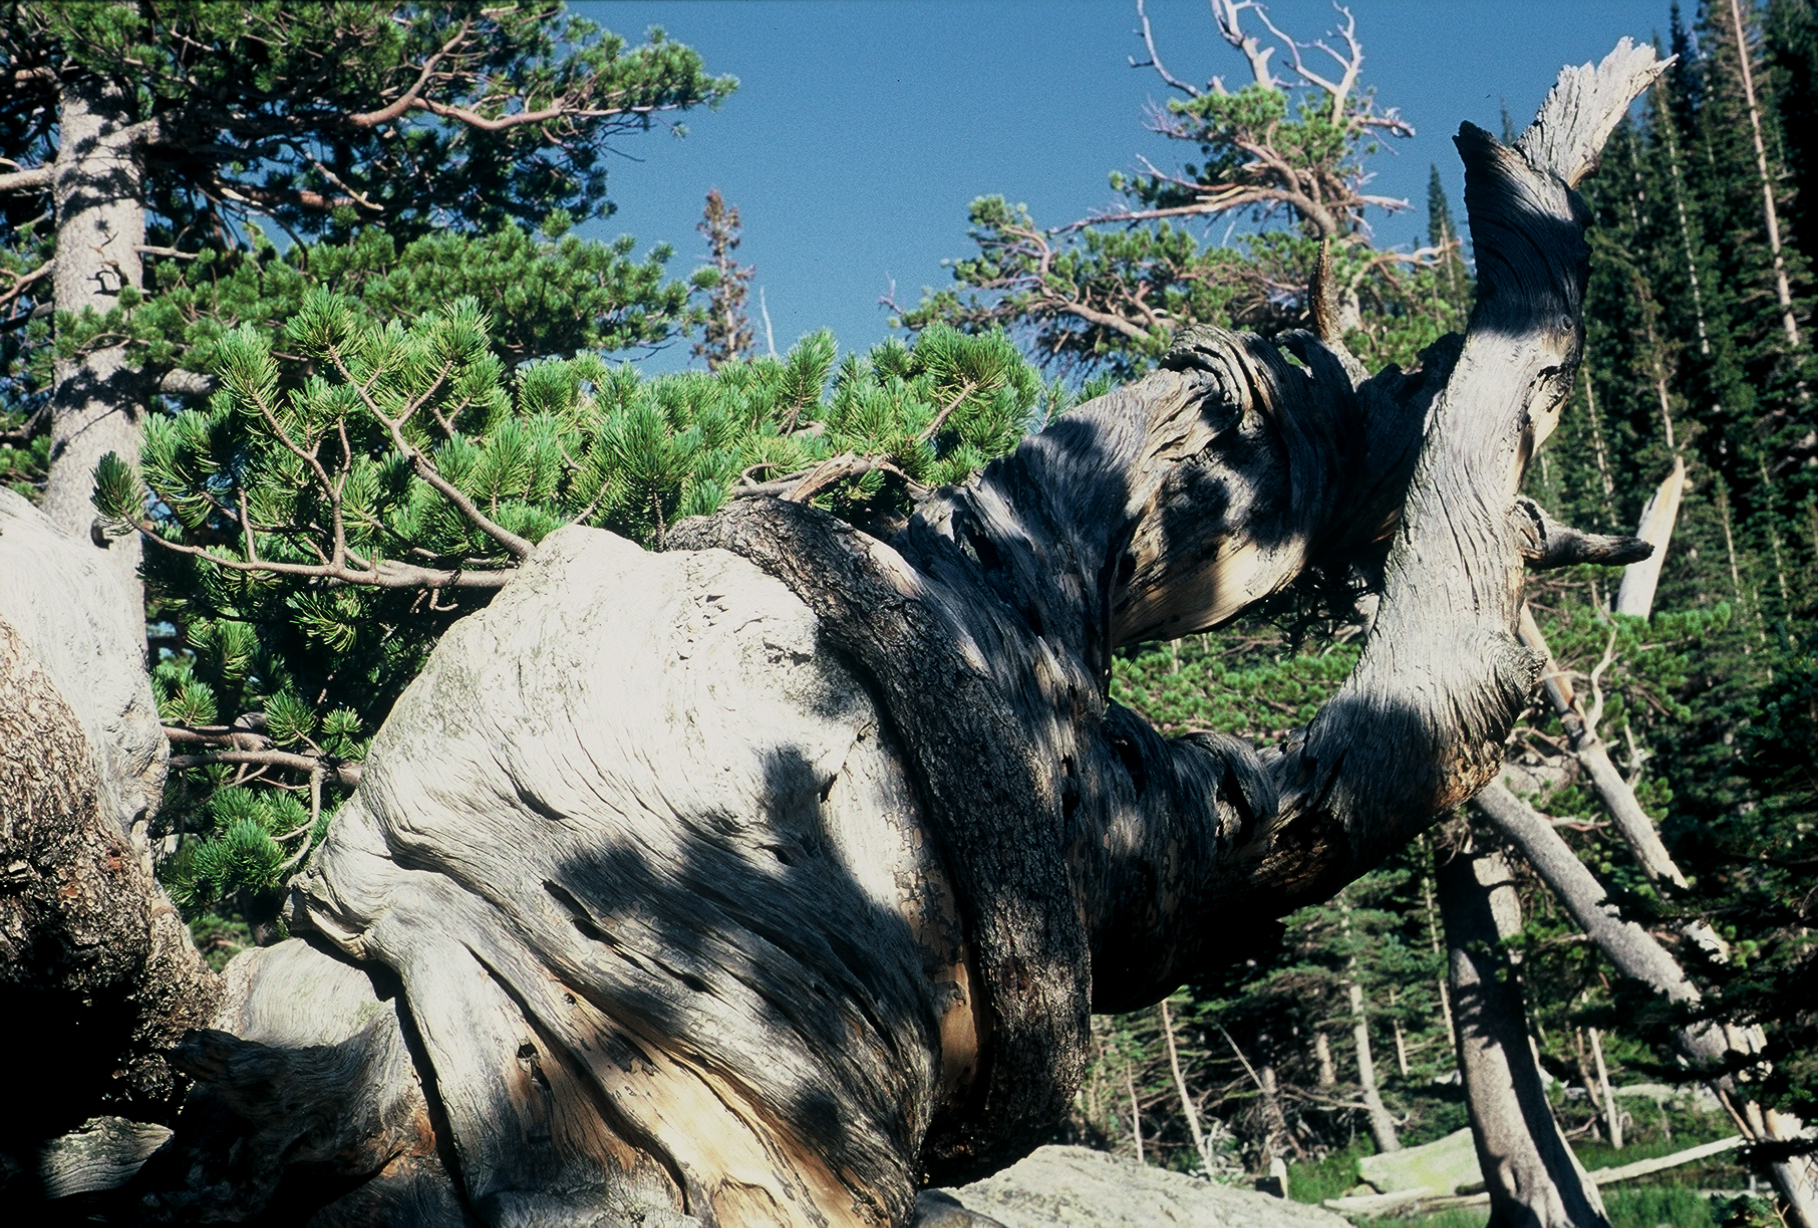
limber pine (Pinus flexilis) – one of the species killed by Cronartium ribicoli; photo by F.T. Campbell

Among the studies available for analysis, reports on plants dominated: 605 focused on plant invasions, 114 on animal invasions, and only 56 on microbial invasions. Among the animals were one study of Adelges tsugae (hemlock woolly adelgid), two studies of Agrilus planipennis (emerald ash borer) and one study each of Lymantria dispar (spongy moth), and Ips pini (North American pine engraver). Studies also addressed earthworms, ants, rats, and feral hogs. Microorganisms included Cronartium ribicoli (white pine blister rust) and several Phytophthora species, including P. agathidicida (kauri dieback), P. alni (affects alders), and P. ramorum (sudden oak death).

Thakur et al. note the skewed taxonomic coverage and say that the low number and narrow taxonomic/ecological variety in the animals and microorganisms probably limit their ability to reach robust conclusions about the impacts of such invasions.

The most consistent negative impact they found is reductions in native plant diversity. While this is not surprising given the studies analyzed, I think it is still important since it counters the widespread sense that plant invasions are somehow less deserving of a robust response.

The authors also detected some broader ecosystem impacts of plant invasions. Plant invasions increased soil organic carbon; soil nitrogen (ammonium and nitrate), and available phosphorus; soil moisture, litter biomass; and emissions of carbon dioxide (CO2), nitrous oxide (N2O), and methane (CH4). The changes in biogeochemical properties might reinforce impacts on native plant communities. The reported increase in greenhouse gas emissions might reflect a bias in the studies so Thakur et al. call for more research to solidify this finding.

High native plant species richness had only a weak overall effect on ecosystem-level impacts. While plant invasions often resulted in higher overall plant species richness, when considering only native community responses, the gain in species numbers did not necessarily indicate conservation benefits. Native plants’ biomass increased after invasion. This might reflect short-term increases in productivity in response to altered resource conditions or structural facilitation, rather than a long-term reversal of competitive exclusion. Finally, the longer the invasive [plant] species had been present, the greater the negative effects on native diversity. However, soil abiotic property impacts weakened over time. In fact, the initial increase in soil organic carbon and total nitrogen disappeared after 6 to 10 years. This development might reflect fertilization of ecosystems by long-established nitrogen-fixing invaders such as non-native legumes.

Traits of non-native plant species related to growth and resource acquisition were overall weak predictors of ecosystem impacts. Thakur et al. consider that this finding reflects the relatively narrow range of specific leaf area exhibited by the plant species studied most commonly.

Consequently, Thakur et al. urge managers to focus on containment and impact mitigation, and to prioritize persistent losses of native plant diversity. When considering abiotic responses that might lessen over time, managers should apply “adaptive monitoring” (which is not defined).

Thakur et al. had greater difficulty determining the impacts of animal and microorganism invasions because of the smaller number of studies. They could not determine the effect of native species richness. The observed decline in soil organic carbon they thought was attributable to the large proportion of studies (9 out of 114) that focused on introduced earthworms. Earthworms reduce organic matter by consuming litter. Mammals were also found to reduce soil organic carbon. Introduced insects had no significant ecosystem effects on soil organic carbon. Non-native animals also increased soil emissions of carbon dioxide and nitrous oxide. The microorganisms included in reviewed studies decreased soil ammonium and increased nitrate, consistent with elevated nitrification. While data on body size of invasive animals were sparse, the authors could determine that larger-bodied species tended to increase soil nitrate while reducing effects on total soil N.

Applying the Results

Thakur et al. report that residence time outperformed other factors as a predictor of invasion impacts. The authors regret the scarcity of long-term studies, especially in the Global South, that could increase our understanding of whether these impacts persist or shift under sustained invasion pressure.

How can scientists apply this information in risk assessments evaluating not-yet introduced species or in deciding what is the appropriate intensity of immediate response to newly detected incursions. Should they give greater weight to others’ studies that focus on long-established invasions by the species in question? Otherwise, this finding seems to largely duplicate the long-established “invasion curve”.

I hope scientists will note that observational studies generally showed stronger impacts than experimental ones, particularly in the case of plant invasions. Perhaps this is true because observational studies better incorporate environmental heterogeneity and longer time spans.

Agrostis stolonifera – one of the plants invading on Prince Edward Island, an Antarctic region island under South African jurisdiction. Photo by Stefan Iefnaer via Wikimedia

Thakur et al. note that one factor they analyzed, “latitude”, incorporates several ecological and anthropogenic components relevant to invasion impacts. One element is the greater native bioidiversity in warmer, lower-latitude, regions. According to the “biotic resistance” hypothesis, greater diversity might make these systems more resistant to bioinvasion. However, the situation is complicated by the fact that temperate regions have also often experienced longstanding and intensive land-use modifications — which are believed to facilitate invasive species establishment and spread. I regret that the authors make no attempt to separate the effects of factors that are anthropogenic from those arising from immutable conditions, e.g., latitude, topography, weather patterns, etc.

Thakur et al. call for more studies that cover a wider geographic range. In addition, the studies should include more experimental designs and explore the relationship between invaders’ traits and impacts — especially regarding animals and microbes.

SOURCE

Thakur, M.P., Z. Gu, M. van Kleunen, X. Zhou. 2025.  Invasion impacts in terrestrial ecosystems: Global patterns and predictors. Science 23 October 2025

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

Threats to Spring

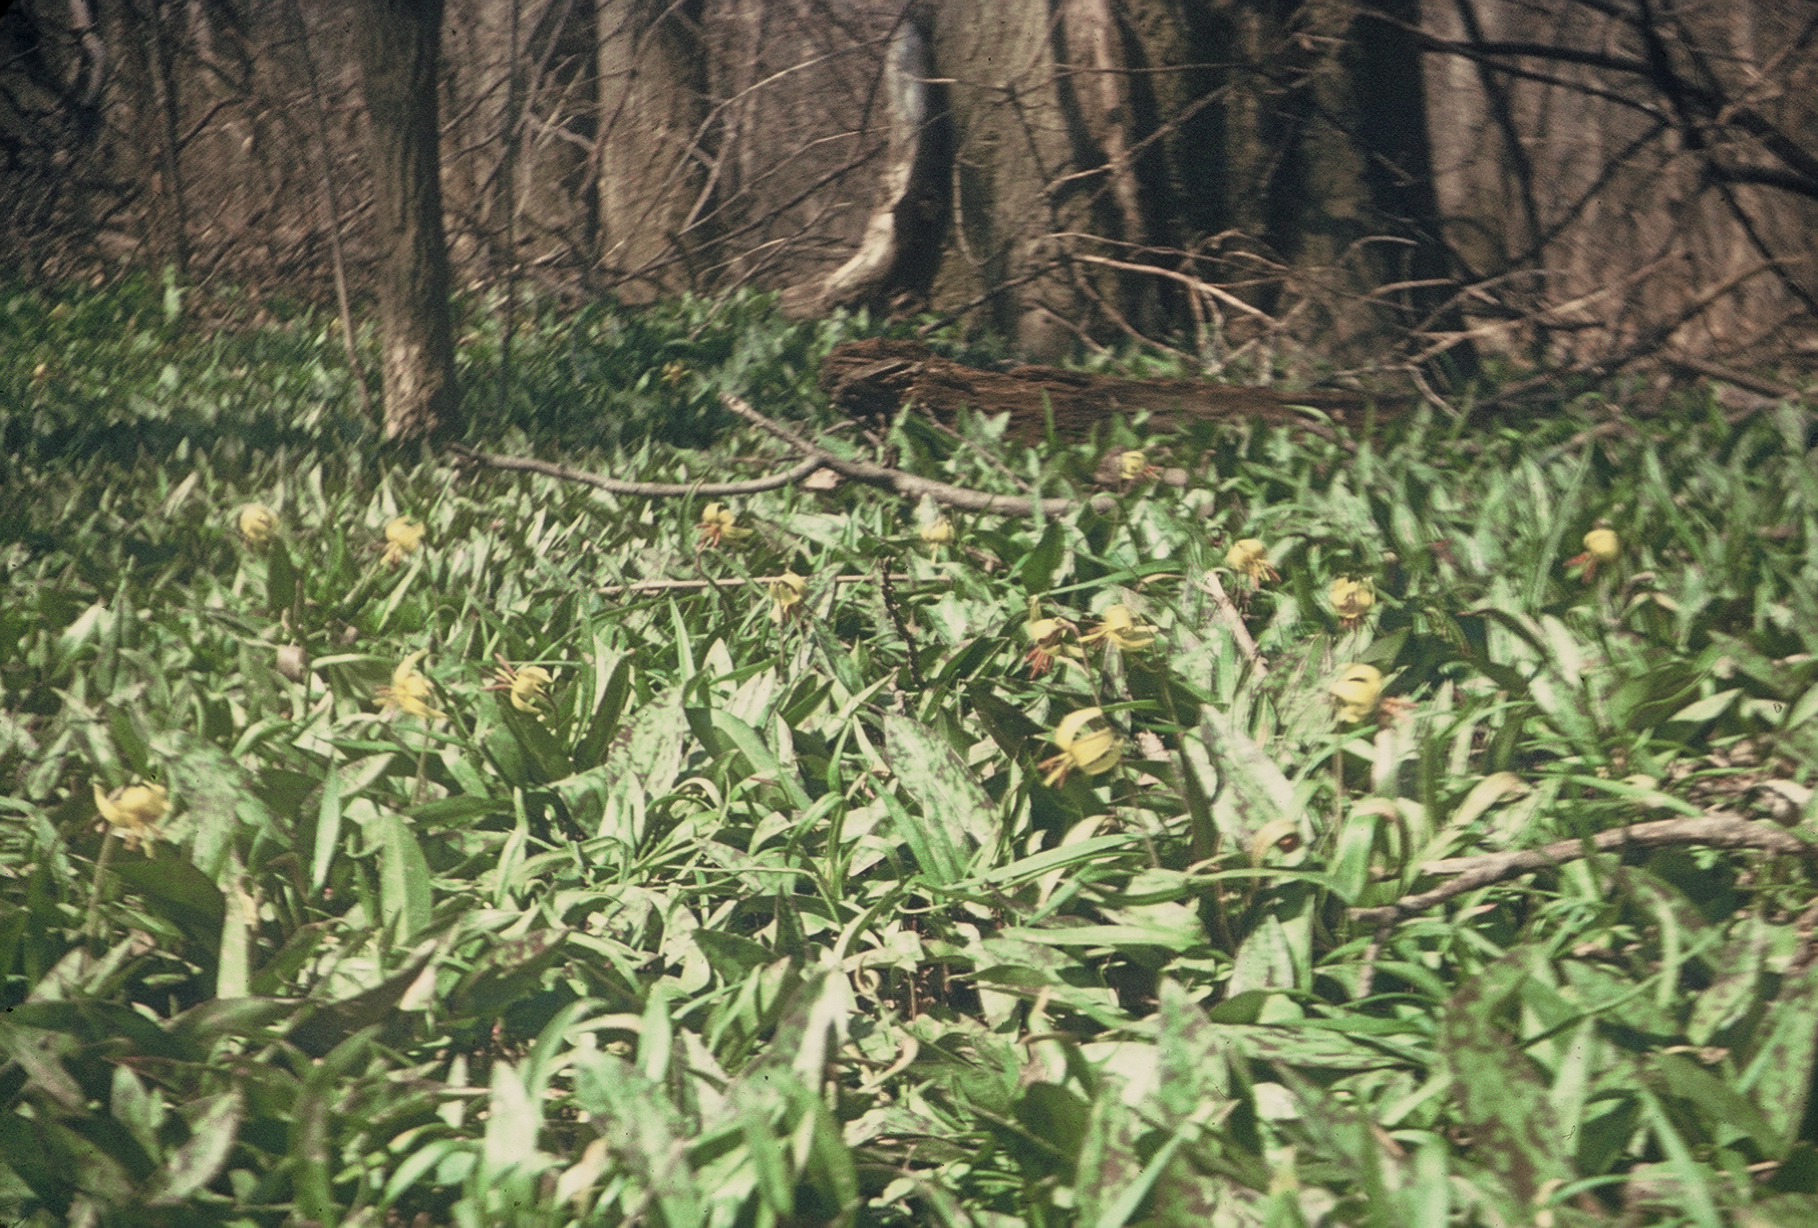
Erythronium americanum dominating herb layer in woods owned by the Institute for Advanced Studies, Princeton, in the 1970s; photo by F.T. Campbell

I fell in love with spring ephemerals in the woods of the Institute for Advanced Studies in Princeton. While the degree I was pursuing had no relationship to birding in the swamp, I spent a lot of time enjoying the woods. At that time, more than 50 years ago, the herbaceous layer was dominated by spring beauties (Claytonia virginica), trout lilies (Erythronium americanum), and violets (Viola species).

Beyond the beauty that delights us (or at least, me!), spring ephemerals are important ecologically. They support specialist pollinators and reduce nutrient losses at a time of year when vegetation cover is low and leaching and runoff rates high.

In the decades since I left Princeton, scientists and nature lovers have observed declines in native understory plant communities. These are predicted to continue due to invasion by plants and worms, worm blogs herbivore pressure by deer, E NPS blog, Blossey blog land use changes, and climate change.

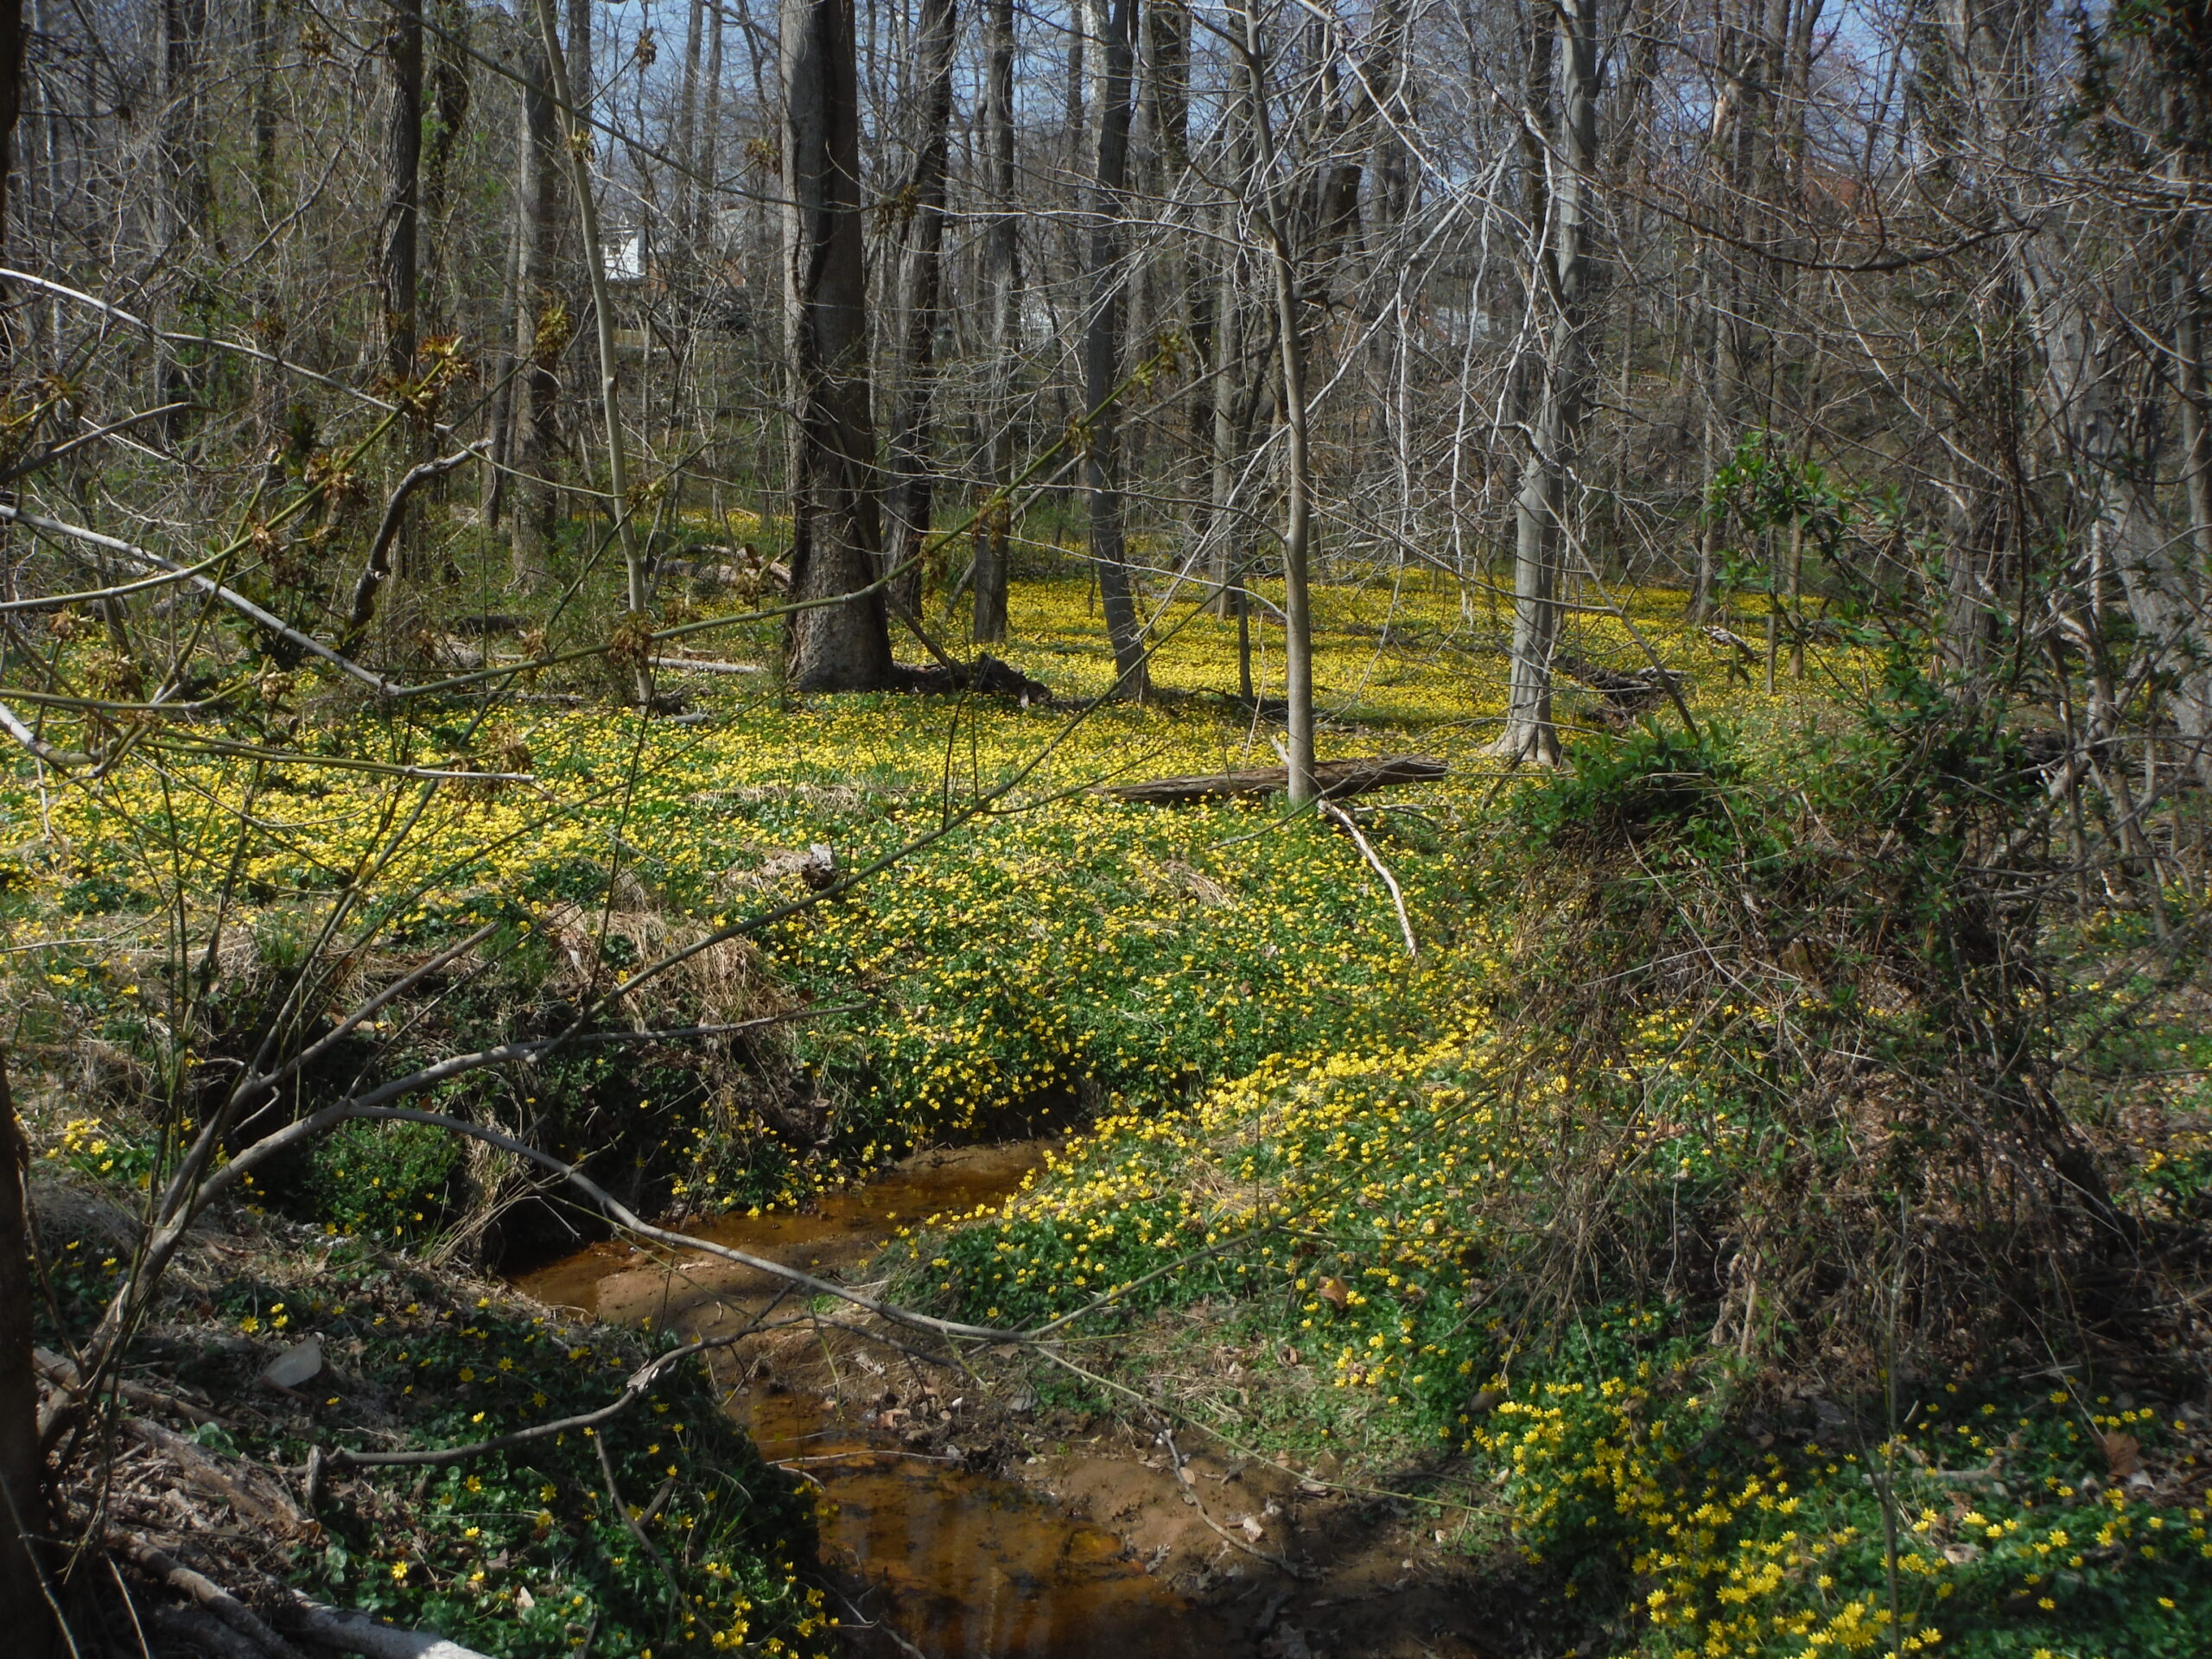
Where I live, in the suburbs of the District of Columbia, these forces are clear. The formerly glorious riparian forests where I walk are overrun by invasive plants. The herb layer is dominated by Japanese stiltgrass (Microstegium vimineum) and – increasingly — lesser celandine (Ficaria verna = Ranunculus ficaria). (I found it interesting that Ficaria began taking over floodplain forests only in the last decades of the 20th century, although it was introduced more than 100 years earlier.) Many invasive shrubs (Rosa multiflora, various Lonicera species. …) and vines (Ampelopsis sp, Orbiculatus, Lonicera japonica, Hedera helix …) compound the problem. While I am not sure whether most earthworms here are native or not, high deer populations certainly are a factor.

Ficaria invasion in Fairfax County, Virginia in 2023; photo by F.T. Campbell

So I rejoice that scientists are studying how one taxon of spring ephemerals, trout lilies – Erythronium species – are coping with individual and combined threats. Gutiérrez and Hovick (full citation at the end of this blog) investigated how two species of Erythronium performed in the absence of a leaf litter layer – with and without competition by Ficaria. They chose to manipulate leaf litter as a proxy for impacts from invasive earthworms and non-native shrubs, especially those with rapidly decomposing leaves.  They refer to others’ studies focused on different spring ephemerals.

Gutiérrez and Hovick found that the absence of leaf litter reduced asexual reproduction (corm biomass) in both Erythronium albidum and E. americanum species by 30%. That is, the absence of leaf litter alone reduced the native plants’ performance. This is alarming because persistent leaf litter has been reduced across much of the deciduous forests of eastern North America as a result of action by invasive earthworms and the rapid decomposition of the leaves of most invasive shrubs.

Trout lilies’ performance declined even more when litter absence was coupled with direct competition from Ficaria. Under those conditions, corm biomass declined by 50%. Impacts by lesser celandine occurred despite these plants’ being smaller than counterparts in nearby woodlands. The reduced size of Erythronium corms was sufficient, in their view, to reduce the likelihood that Erythronium would flower to nearly zero. This has clear implications for the long-term population viability of Erythronium andtheir specialist pollinators.

 Gutiérrez and Hovick conclude restoration of these floodplain forests’ herb layer must incorporate management strategies that not only reduce Ficaria’s presence but also restore leaf litter.

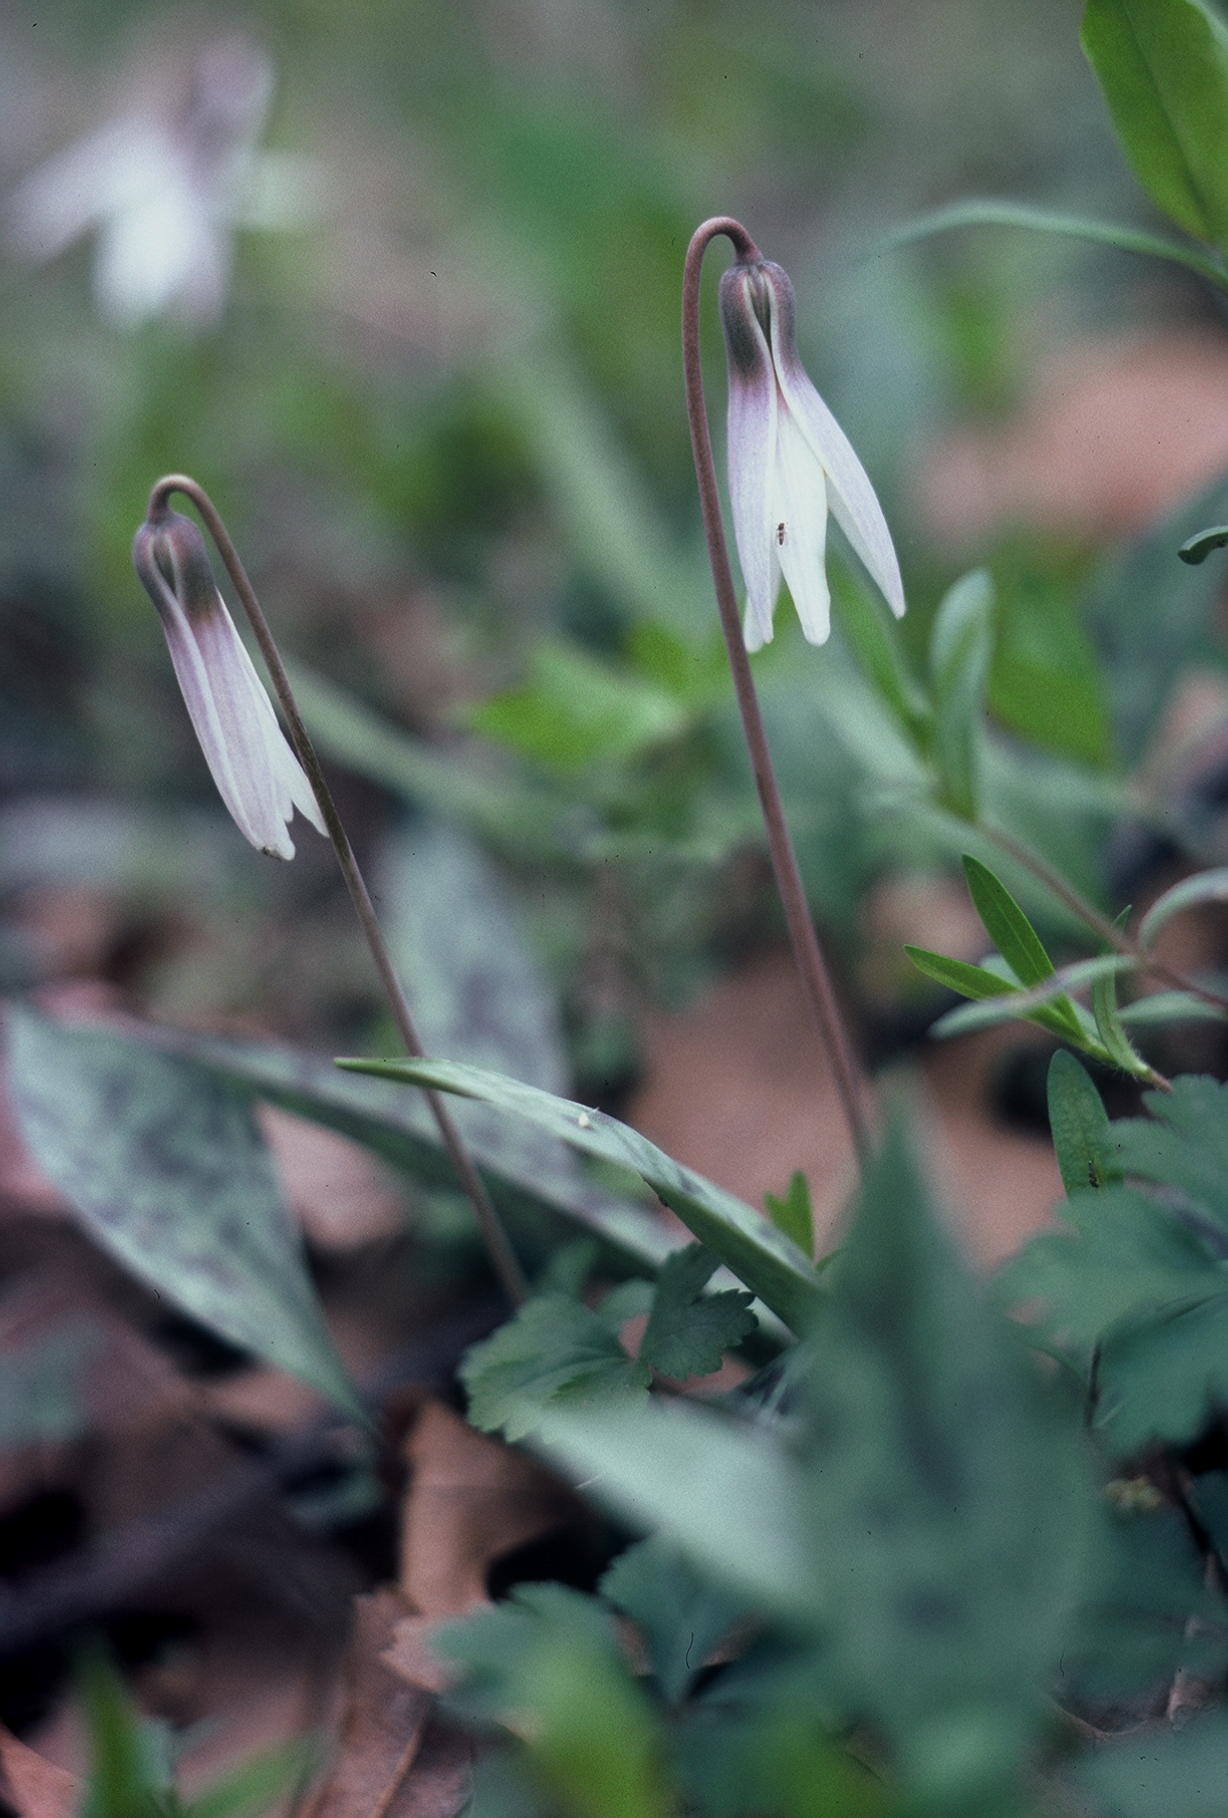
Erythronium albidum along Accotink Creek in Fairfax County, Virginia; photo by F.T. Campbell

Underlying Factors

Native spring ephemerals in eastern North America evolved to emerge through litter layers in early spring. The litter layers impose both costs and benefits. In response to shading by leaf litter, Erythronium produces larger petioles compared to same-sized leaves, thus reducing the proportion of resources allocated to building photosynthetic tissue. In these cases, the corms that both perpetuate the individual and carry out asexual reproduction are smaller.

On the other hand, leaf litter increases moisture retention and reduces frost damage by buffering soil temperatures. While these results were seen in their experiment, Gutiérrez and Hovick believe the benefits are greater in nature than demonstrated in the study using potted plants. Leaf litter also increases nutrient availability, directly by increasing supply and indirectly by facilitating fine root growth. In this context, they note that their experiment used litter composed of just two tree species — red oak (Quercus rubra) and red maple (Acer rubrum). This narrow sample probably failed to capture the varied properties of other tree species’ litter and associated microbial activity.

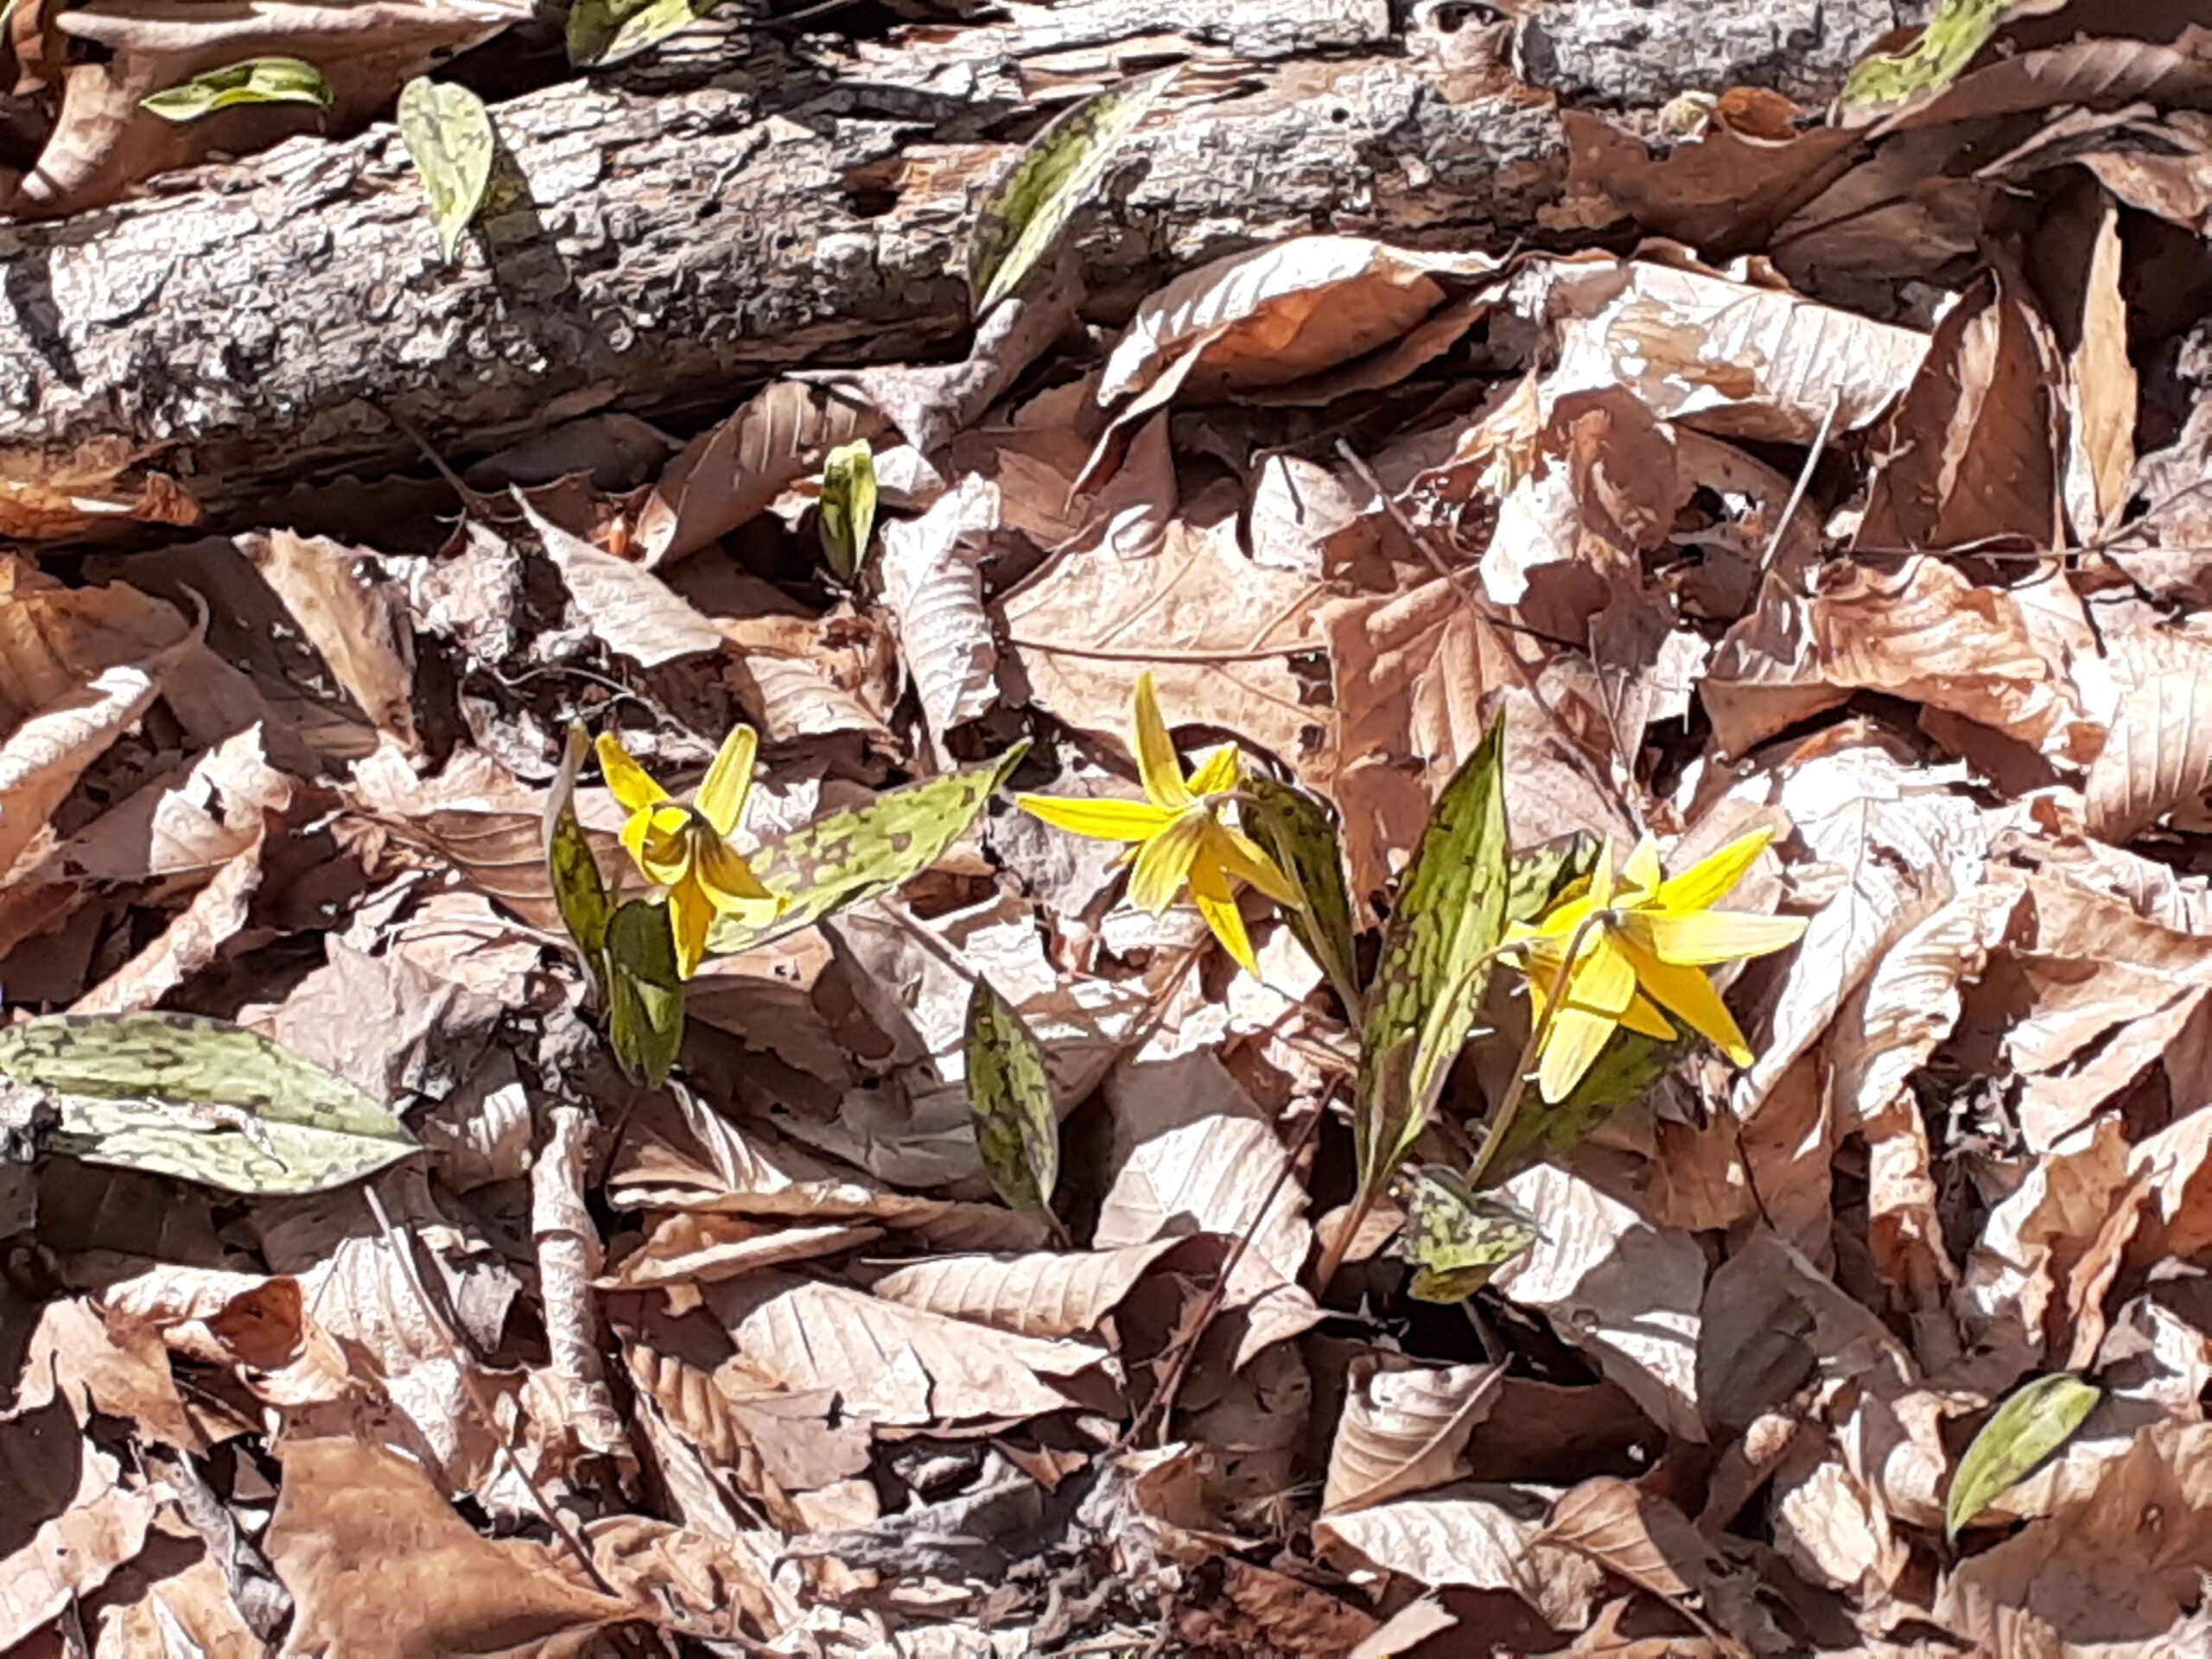
Erythronium americanum along Pohick Creek; photo by F.T. Campbelle

Plants in the Erythronium genus reproduce primarily asexually through producing runners that form corms. The parent corm and runners disintegrate before summer dormancy; the offspring corms persist. Some individuals do not reproduce asexually; they simply replenish their own corm.

The few previous studies give mixed results regarding lesser celandine’s impacts on co-occurring native herbaceous plants (see the summaries in Gutiérrez and Hovick). The authors do not explicitly say whether lesser celandine is usually associated with low litter levels, but that appears to be the implication. They do say that it is not clear whether lesser celandine drives leaf litter loss by altering soil physiochemistry and microbial activity. Or, rather, that it simply performs well when leaf litter is absent.

Where lesser celandine and Erythronium co-occur at high densities, the former’s biomass per square meter can be more than an order of magnitude higher than Erythronium. Gutiérrez and Hovick suggest that competition between the species is primarily belowground. They cite their finding that by the time Erythronium shoots matured, lesser celandine roots occupied most of the belowground pot volume. They expect belowground competition in forests to be even more pronounced because of accumulated lesser celandine root biomass.

Aboveground, the principal factor appears to be the necessity for trout lilies to grow longer petioles to raise their leaves above lesser celandine rosettes, perhaps starving leaf formation. Since leaves are the plant’s photosynthetic organ, this tradeoff could ultimately result in fewer resources returned to the corm for future growth and reproduction. Although Gutiérrez and Hovick also mention that lesser celandine competition might delay Erythronium emergence and flowering, they do not discuss that.

A factor not mentioned by Gutiérrez and Hovick is the probability that Ficaria verna is allelopathic. See the article by Kendra Cipollini listed as a source at the end if this blog.

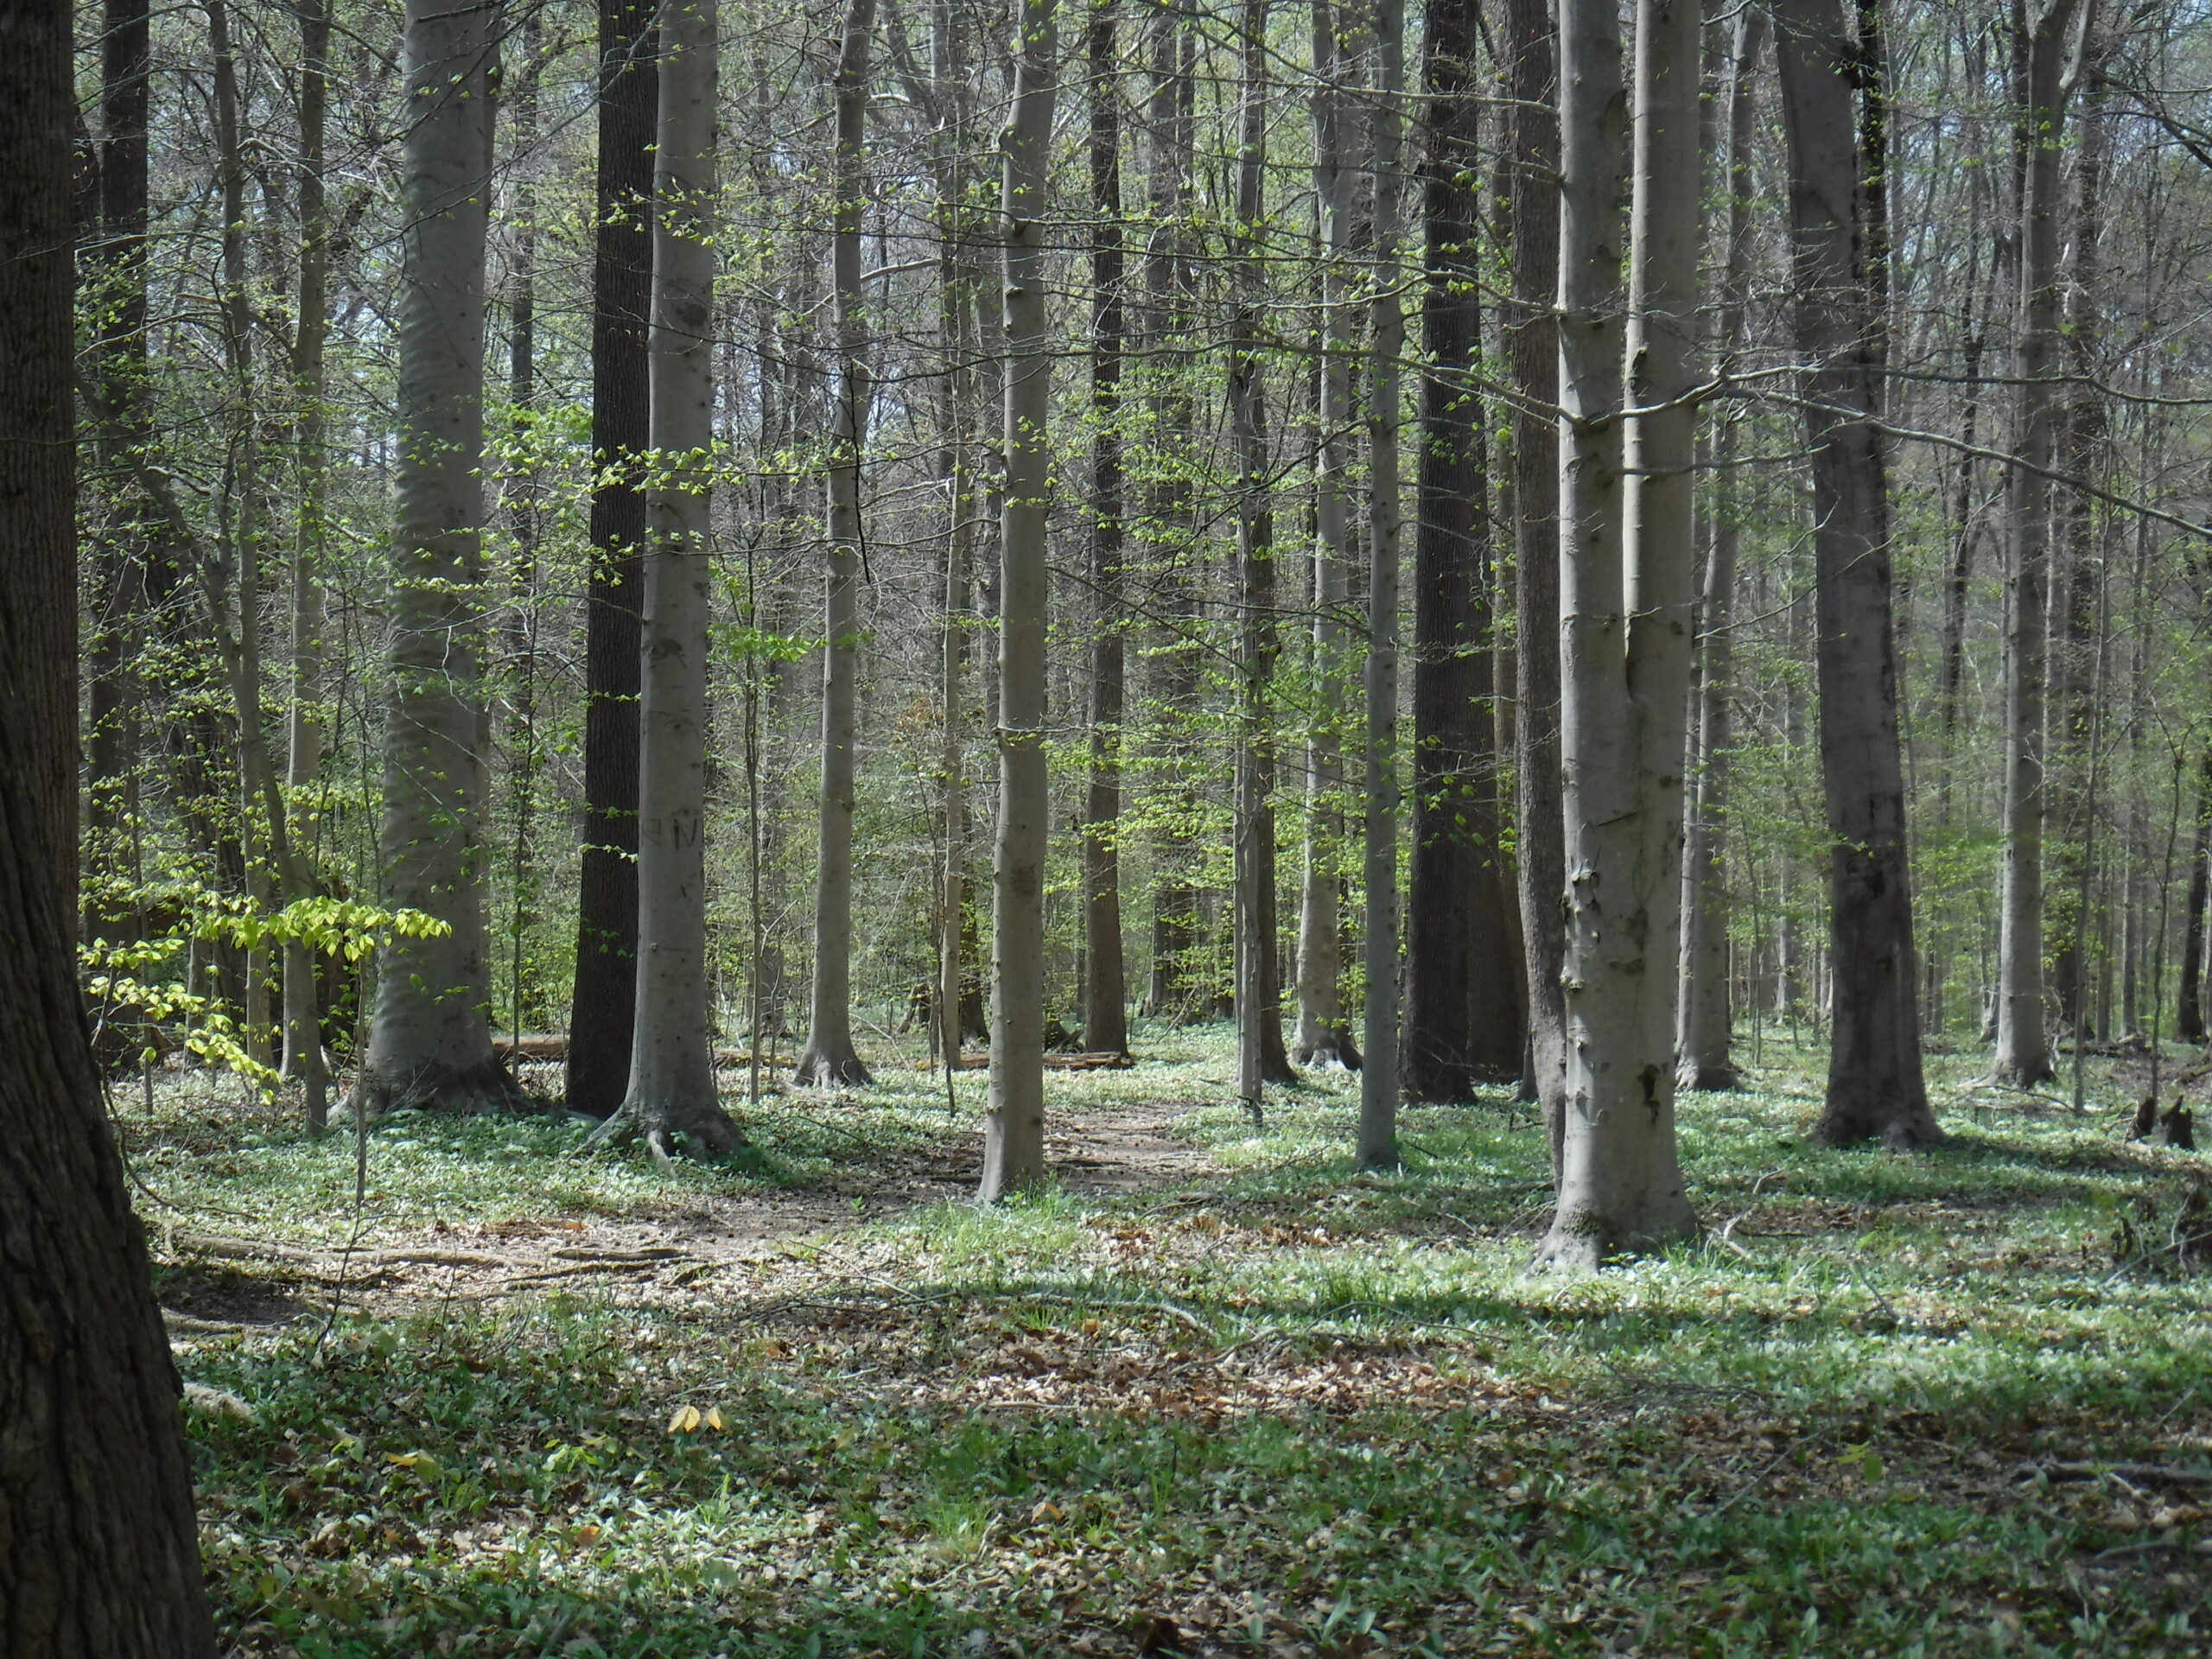
one of the few floodplains in Fairfax County still dominated by native herbs – Pohick Creek in the Burke area of Fairfax County, Virginia. Note the prevalence of beech in the canopy and subcanopy! photo by F.T. Campbell

Details of Impaired Performance of Erythronium

At the time of senescence, Erythronium plants grown in pots with leaf litter were nearly twice as large as those grown in bare soil conditions. One-third of their offspring corms grew to be larger than the putative biomass threshold for flowering. Only 9% of corms of plants grown in bare soil and 2% (one individual) of those grown with lesser celandine did. As noted above, corms developed by Erythronium grown in the presence of Ficaria actually lost biomass. This is the basis for their conclusion that there would be almost no sexual reproduction the following year where litter was absent and lesser celandine present.

Gutiérrez and Hovick think the principle mechanisms by which leaf litter affects performance of Erythronium plants is by buffering temperature ranges and increasing moisture retention. Indeed, they found that daily temperature ranges and maxima of soil in pots with bare soil or lesser celandine plants were both higher than temperatures under leaf litter. Reducing temperature maxima could be especially important with the increasing frequency and intensity of late-spring heatwaves associated with climate change. Absence of leaf litter advanced trout lily’s shoot emergence, flower emergence, and petal opening by 14 or more days.

This change might expose the plants to increased risk of frost damage. These dynamics will be system-specific, especially with complications added by climate change. However, Therefore, Gutiérrez and Hovick encourage future research to explore species-specific litter effects on spring ephemerals.

Broader Implications

Their findings regarding these two species of spring ephemerals prompt Gutiérrez and Hovick to assert that negative impacts from invasive plant species might be especially underestimated in spring ephemeral communities due to the combination of their short period of annual aboveground activity and tendency towards long lives. Changes might be very subtle over short timeframes.

They add that it is important to learn the role different conditions might play in the futures of related species. The two species’ ranges largely overlap, but E. americanum extends into the extreme southeast and northeast, E. albidum into the prairie states. Although these species’ respond to loss of leaf litter and lesser celandine invasions in similar ways, the fact that E. albidum occurs in areas of higher soil moisture makes it more vulnerable to negative population-level impacts from lesser celandine invasions.

Note about additional threats

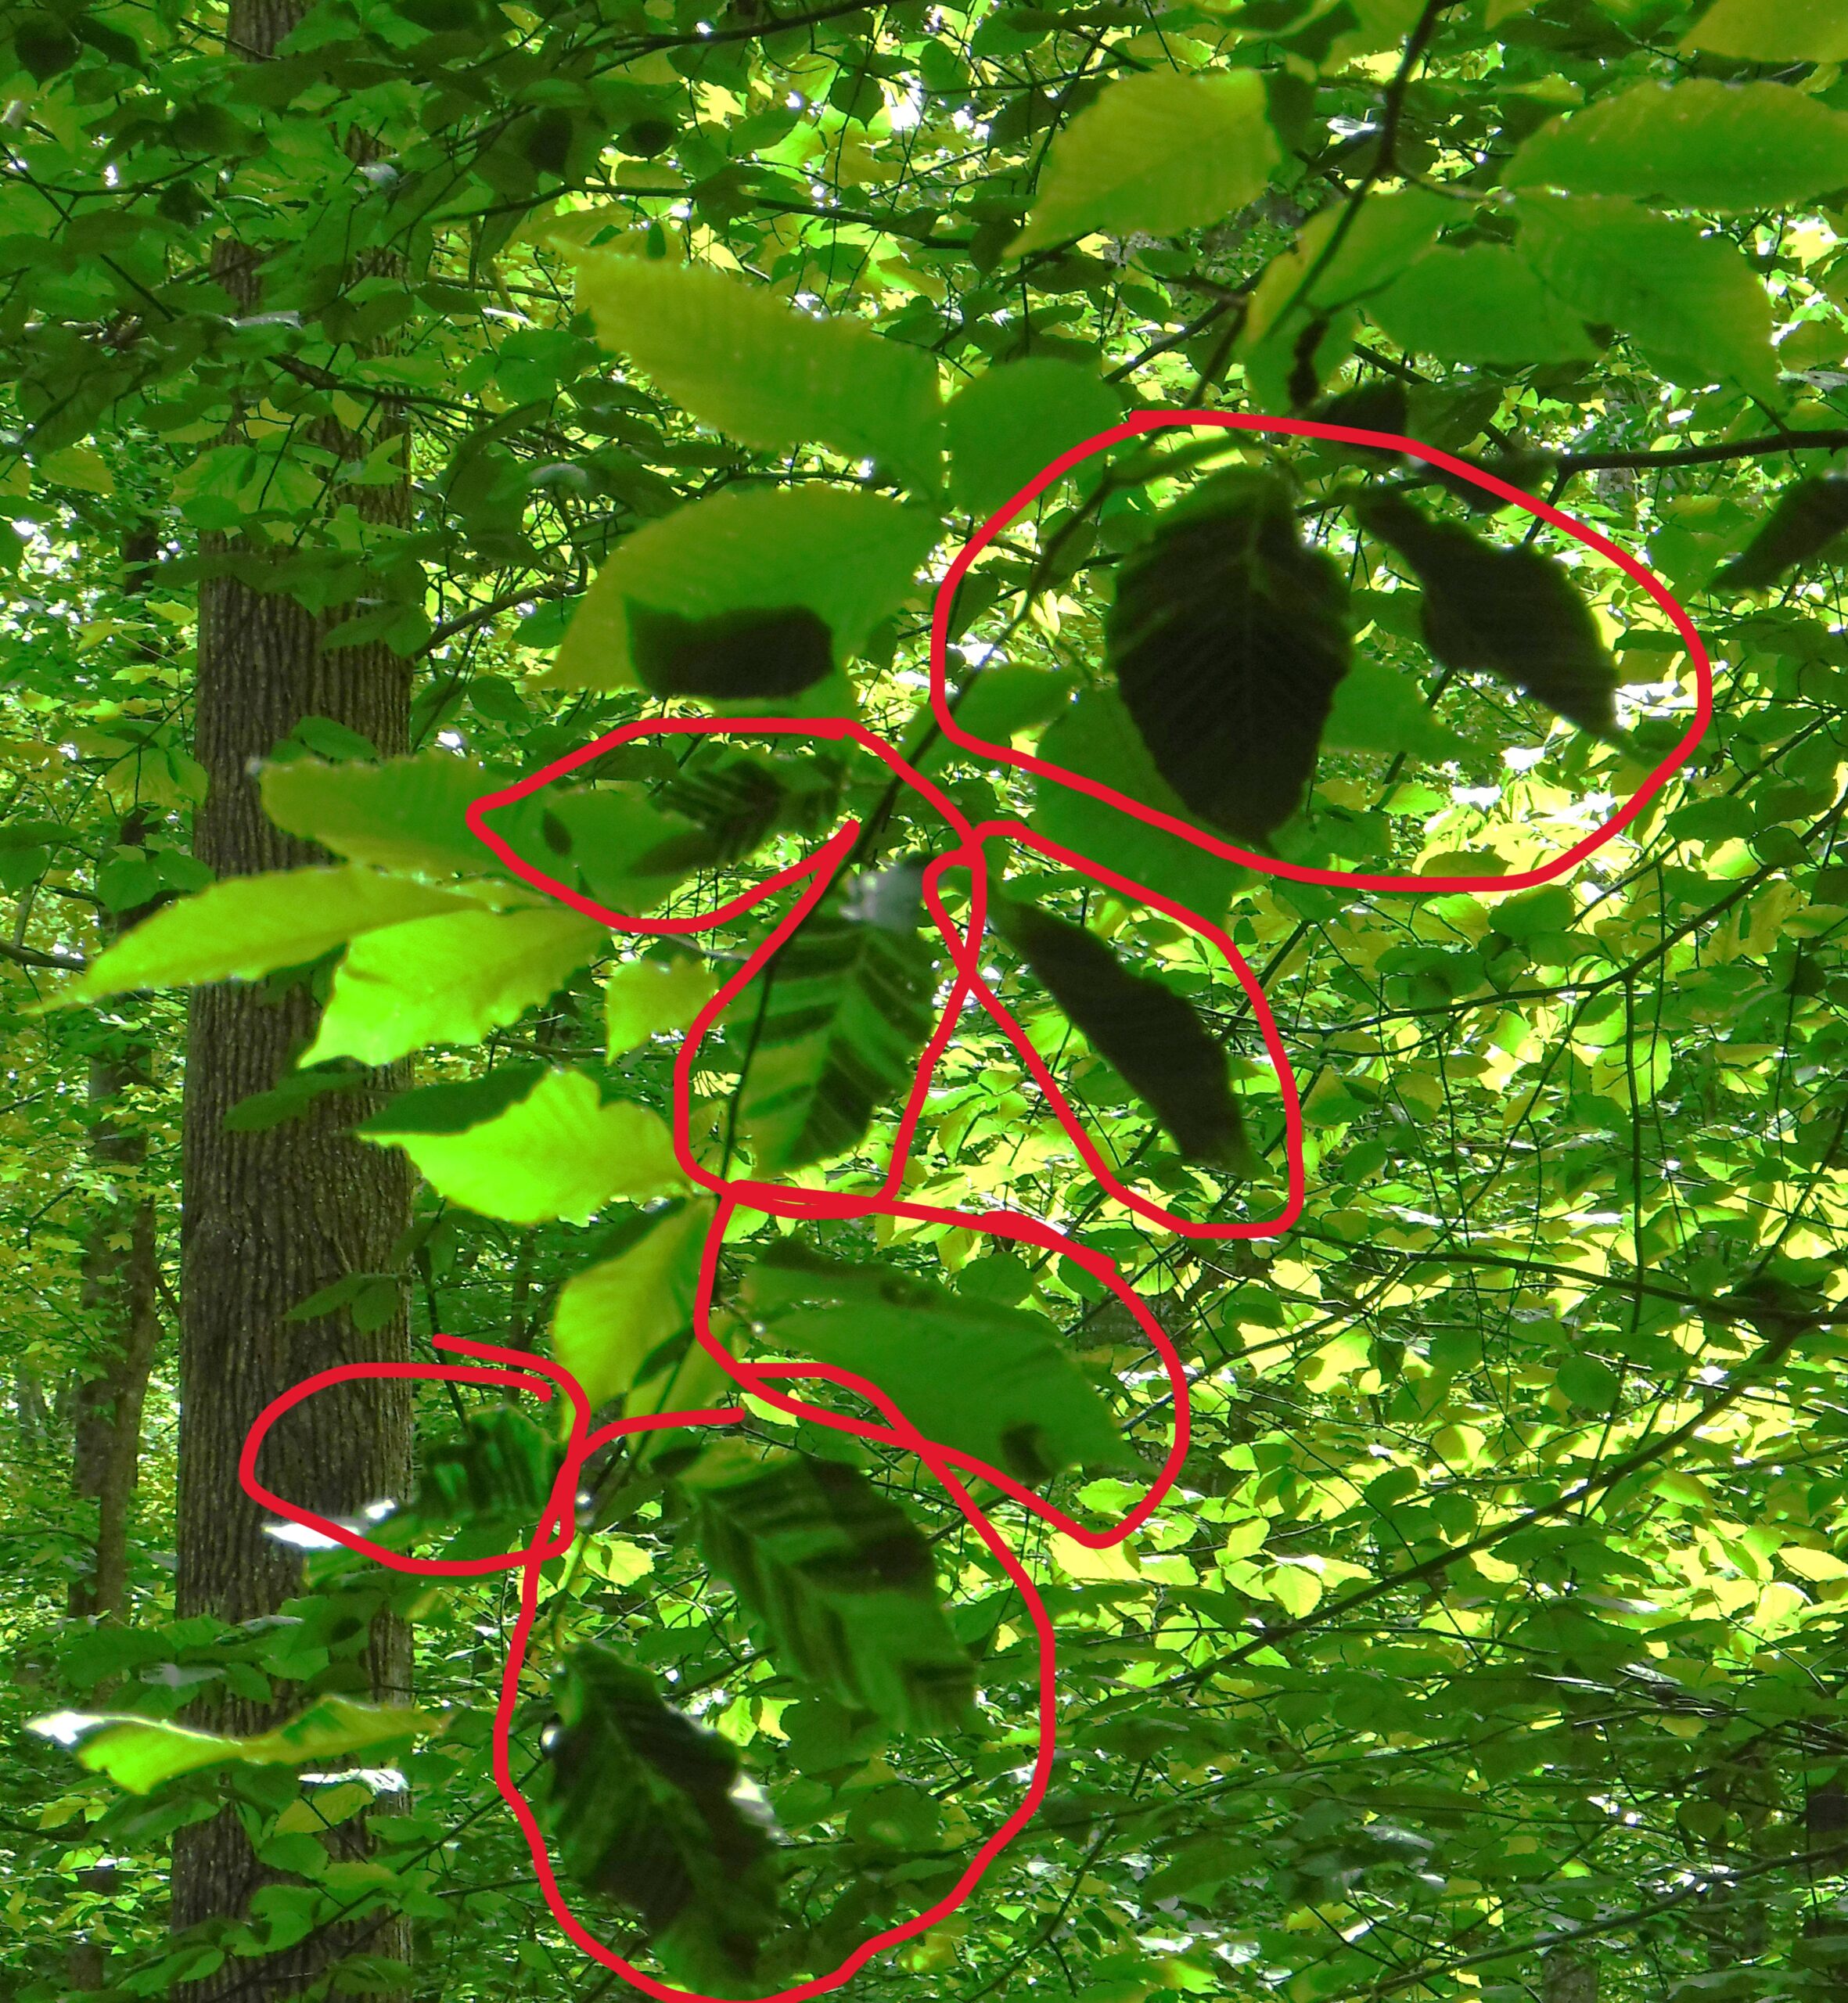
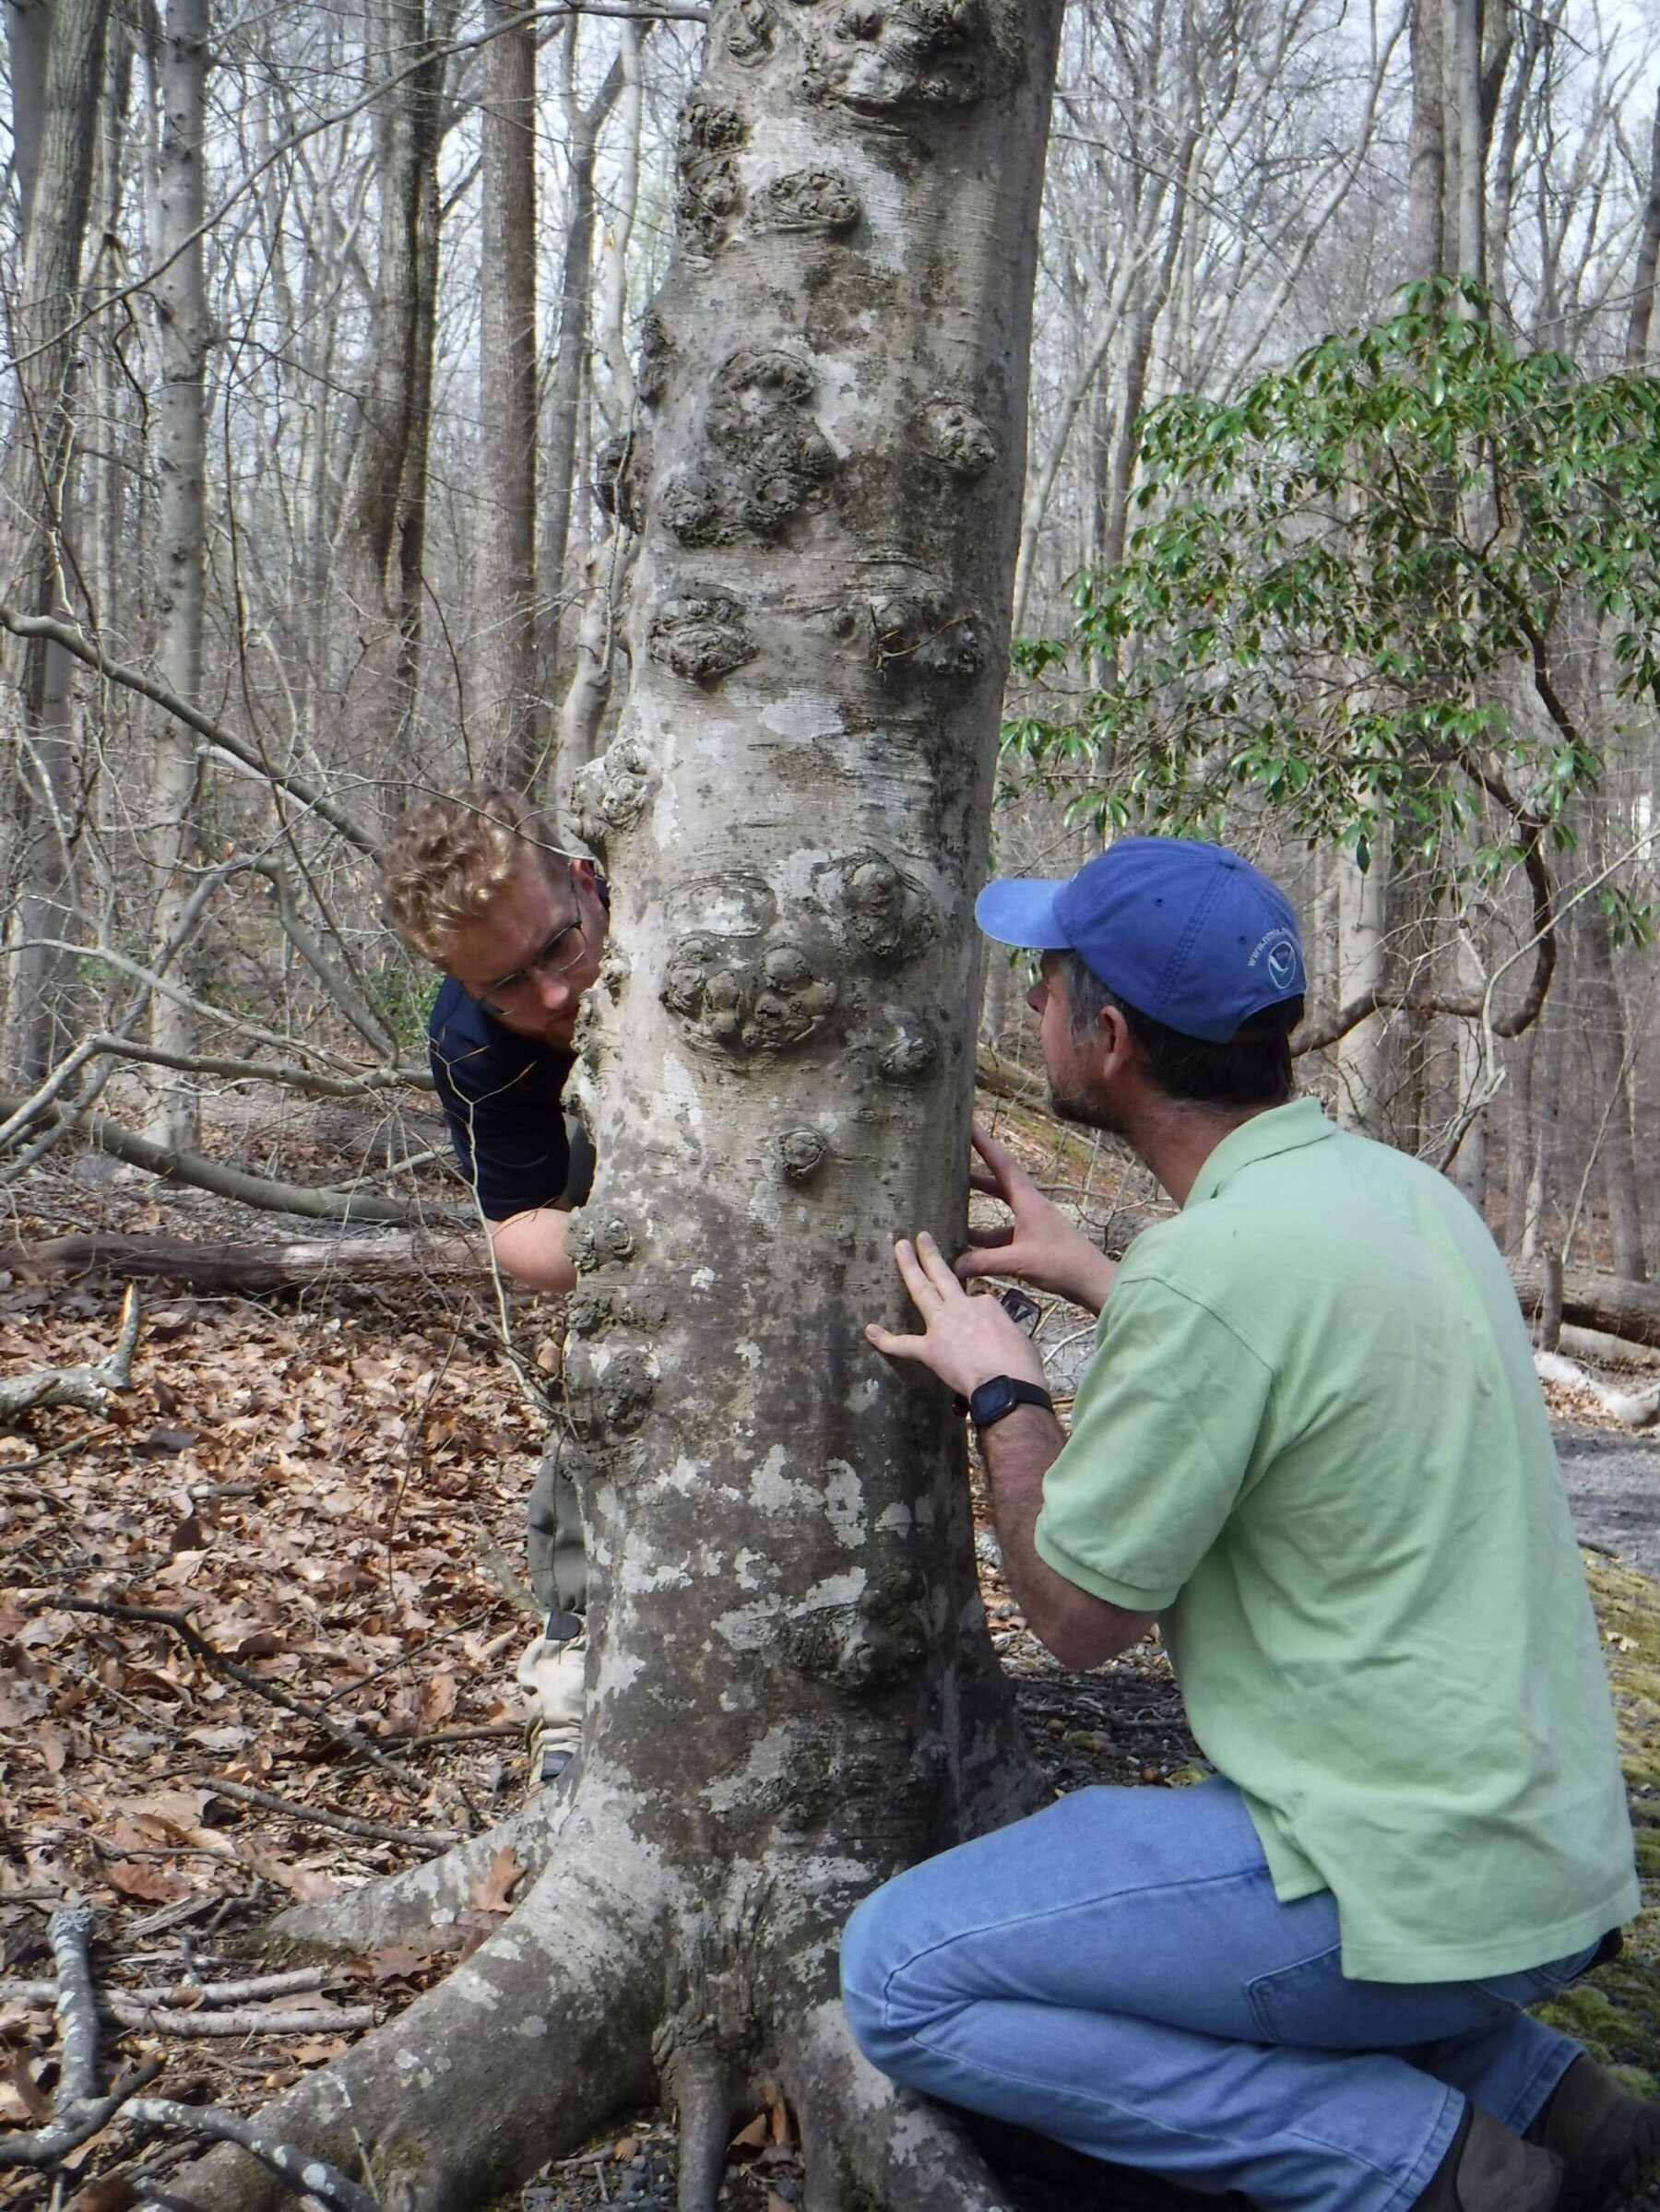
Most of the photos of Erythronium americanum in this blog were taken along a particular creek in Fairfax County, Virginia. Ficaria has just begun to invade this area (see photo above); deer are plentiful. These plants face another bioinvasion: beech leaf disease has arrived. Widespread mortality of the predominantly beech understory will presumably open areas to more light, probably spread of the extant invasive plants.

beech in Fairfax County, Virginia with symptoms of beech leaf disease; photo by F.T. Campbell

SOURCES

Cipollini, K. and K.D. Schradin. 2011. Guilty in the Court of Public Opinion: Testing Presumptive Impacts and Allelopathic Potential of Ranunculus ficaria” 

Gutiérrez, R.G. and S.M. Hovick. 2025. Compounding negative effects of leaf litter absence and belowground competition from an invasive spring ephemeral on native spring ephemeral growth and reproduction. Biol Invasions (2025) 27:213 https://doi.org/10.1007/s10530-025-03668-4


Call for new approach to biological conservation – integrating bioinvasion

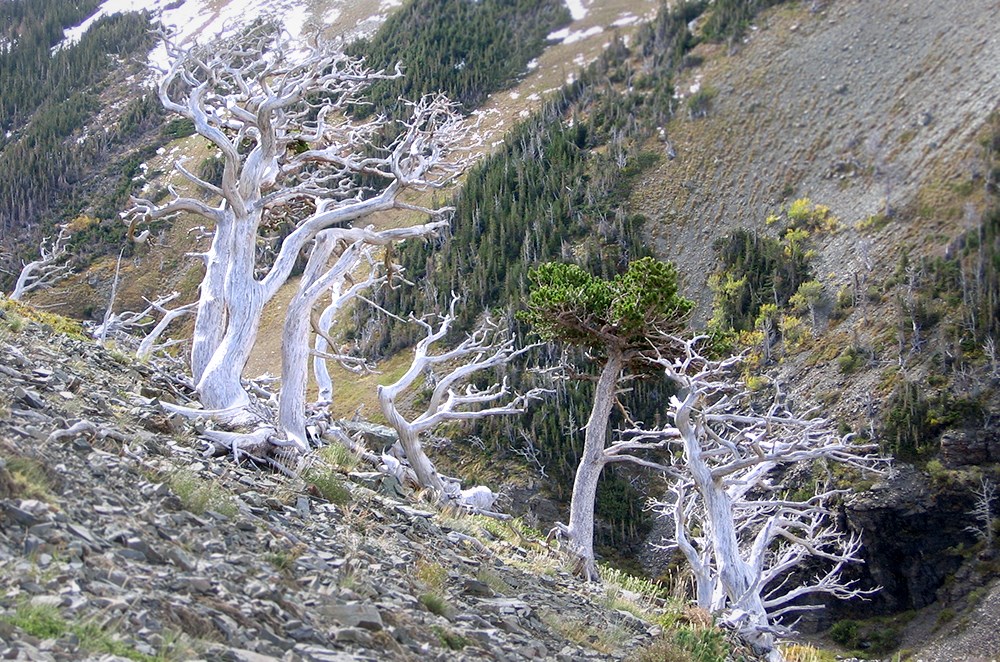
whitebark pine in Glacier National Park killed by white pine blister rust

The Kunming-Montreal Global Biodiversity Framework (KMGBF) is a major global policy driver around the world for more effective action to preserve biodiversity from current and future threats. (However, the United States has not joined the underlying treaty, the Convention on Biological Diversity (CBD). So its importance is probably less in the United States than in countries that take part.) This relatively new Framework was adopted at the 15th Conference of the Parties (COP) of the CBD in December 2022 after four years of negotiations. However, cynics note that the 196 countries that are parties to the CBD have rarely met previous ambitious goals set at earlier COP.

Hulme et al. have just published a paper [full reference at the end of this blog] addressing how invasive species and this Framework’s target may interact. They note that conserving biodiversity costs money. Many of the countries hosting diverse and relatively intact ecosystems lack sufficient resources, capability, or robust governance structures for this conservation.

The Kunming-Montreal Global Biodiversity Framework sets out ambitious global targets to reduce biodiversity loss by 2030 so as to maintain the integrity of ecosystems and their constituent species. Of the 23 targets, one – Target 6 – addresses bioinvasion. Countries endorsing the CBD have committed to eliminating, minimizing, reducing and/or mitigating invasive species’ impacts on biodiversity and ecosystem services. This is to be accomplished by identifying and managing introduction pathways; preventing introduction and establishment of priority invasive species; reducing rates of introduction and establishment of known or potential invasive species by at least 50% by 2030; and eradicating or controlling invasive species, especially in priority sites.

I rejoice that the CBD parties have recognized invasive species as a major driver of biodiversity loss in terrestrial and marine ecosystems. I wish conservation organizations’ and funders’ activities clearly reflect this finding.

This is the challenge raised by Hulme et al.: countries must integrate efforts to counter bioinvasions into overall conservation programs. Success in curbing bioinvasion depends upon achieving almost all other KMGBF targets. And this is a two-way street: the more holistic approach offers greater likelihood of successful biodiversity conservation.

The same authors point out that some of the 22 other targets address rapidly evolving introductory pathways e.g.,

  • Target 15 – increasing international and domestic tourism;
  • Target 12 – encroachment of urban areas near protected areas;
  • Target 10 – development of intensive agriculture or aquaculture systems near protected areas;
  •  Target 7 – species rafting on plastic marine pollutants; and
  • Target 8 – growing risk from species shifting ranges in response to climate change.  
pallet graveyard behind camp store & snack bar art Lake MacDonald, Glacier National Park; photo by F.T. Campbell

Other targets relate to management of established invasive species, e.g.,

  • Target 1 – planning and priority-setting for allocation of limited resources among the various threats to biodiversity;
  • Identifying factors that pose risks to highly-valued species, e.g., threatened species (Target 4) and species that provide important ecosystem services (Target 11);
  • Target 19—obtaining necessary financial resources.  

A final group of targets are intended to guide all conservation efforts. These goals include integrating biodiversity concerns in decision-making at every level (Target 14); reducing harmful economic incentives and promoting positive incentives (Target 18); and several targets addressing issues of equity, benefit sharing, and access to information.  Hulme et al. assert that the threat posed by bioinvasions must be incorporated into policies, regulations, planning and development processes and environmental impact assessments across all levels of government.

Hulme et al. decry an imbalance as to which KMGBF targets have been the focus of attention from governments, conservation organizations, and media. These stakeholders have concentrated on

  • Target 3, which calls for extending legal protection to 30% of lands and waters by 2030;
  • Target 4, which promotes maintaining genetic diversity within and among populations of all species;
  • Target 7,  which encourages reducing harmful pollution;
  • Target 15, which urges businesses to decrease biodiversity risks arising from their operations; and
  • Target 21, which advocates ensuring equitable and effective biodiversity decision-making.

Even when stakeholders have looked at Target 6, they have focused primarily on how to quantify the numbers of species being introduced to novel ecosystems. Hulme et al. argue that conservationists should instead concentrate on the challenge of achieving the target. They note that bioinvasion is worsening despite implementation of many long-term management programs. As they note, numbers of introduced species globally have increased, these species are occupying larger geographic areas, and the species’ measured impacts have risen to astounding levels (see my previous blog about new cost estimates). This same point was made two years ago by Fenn-Moltu et al. (2023) [full citation at the end of this blog]; they found that the number of invasive species-related legislation and treaties to which a country adheres did not relate to either the number of insect species detected at that country’s border or the number of insect species that had established in that country’s ecosystems.

As conservationists, Hulme et al. remind us that not all damages are monetary: invasive species threaten more than half of all UNESCO World Heritage Sites.

Hulme et al. say achieving Target 6 presents several scientific challenges – most of which have been discussed by numerous other authors. Introduction pathways are changing rapidly. There is great uncertainty regarding current and especially future propagule pressures associated with various pathways. Information about particular species’ impacts and where they are most likely to be introduced is insufficient. Management costs are routinely underestimated. Perhaps most challenging is the need to judge programs’ effectiveness based not simply on outputs (e.g., number of acres cleared of weeds) but on outcomes in relation to reducing the subsequent impact on biodiversity and ecosystem services.

I note that several environmental organizations endorsed a “platform” that discussed this last point a decade ago. [I have rescued the NECIS document from a non-secure website; if you wish to obtain a copy, contact me directly through the “comment” option or my email.] Unfortunately, the coalition that prepared this document no longer exists. Even when conservation organizations have invasive species efforts, they are no longer attempting to coordinate their work.

APHIS inspecting imported plants

I greatly regret that Hulme et al. continue a long-standing misrepresentation of international border biosecurity controls as consisting primarily of inspections — of imported commodities, travellers, and associated transport conveyances. I have argued for decades that inspections are not effective in preventing introductions. See Fading Forests II Chapter 3 (published in 2003); Fading Forests III Chapter 5 (published in 2014); “briefs” describing pathways of introduction prepared for the Continental Dialogue on Non-Native Forest Insects and Diseases – in 2014 and in 2018.    

 The weaknesses of visual inspection are especially glaring when trying to prevent introductions via wood packaging material and living plants — also here.

Hulme et al. propose a politically astute approach to finding the resources to strengthen countries’ efforts to curtail invasive species’ spread within their borders.  Recognizing that no country has unlimited resources to allocate to managing invasive species, they suggest concentrating slow-the-spread efforts on preventing damage to legally protected areas. Furthermore, authorities should avoid designating as new “protected areas” places that are already heavily invaded – or at risk of soon becoming so. As they note, programs aimed at protecting these areas often engage conservation stakeholders, decision-makers, even potential non-governmental donors. In other words, there is a foundation on which to build.

To buttress their argument, Hulme et al. cite evidence that bioinvasions threaten these areas’ integrity. For example, Cadotte et al. (2024) found that bioinvasion is one of most frequently identified threats identified in a survey of 230 World Heritage sites; and that they pose a greater degree of concern than other threats to biodiversity. They reiterate that managing invasive species is one of the most effective interventions aimed at protecting biodiversity.

The task remains complex. Hulme et al. note that accurate information about pressure caused by invasive species is not easily quantified using remote sensing. It requires expensive on-the-ground data collection. Even current methods for ranking invasive species have crucial gaps regarding species’ potential impact and the feasibility of their control. Choosing management strategies also requires assessing potential unintended effects on biodiversity and other GBF Targets, e.g., pollution from pesticides (Target 7).

Still, the context remains: successful management of bioinvasions to support the integrity of protected areas depends on the integrative approach described above.

Hulme et al. note a contradiction within the Kunming-Montreal Global Biodiversity Framework: Target 10 calls for the agriculture, aquaculture, and forestry industries to adopt sustainable practices, but doesn’t raise the issue of these sectors’ role in the introduction and spread of invasive species. They say guidelines have been developed for sustainable forestry production. These guidelines recommend that commercial plantation forests not plant non-native tree species within 10 km of a protected area. Hulme et al. also suggest applying a “polluter pays” fine or bond to forestry businesses that use invasive species without sufficient safeguards to prevent escape. These funds could be accessed to support invasive species management in protected areas, particularly surveillance. (Target 19 mandates obtaining more funds for this purpose).  They add that these aquaculture, agriculture, horticulture and forestry sectors should take action to prevent the local feralization of alien crops and livestock.

Target 8 calls for minimizing the impacts of climate change on biodiversity. Hulme et al. note numerous scientific challenges here, including understanding how specific ecosystems’ and native species’ are vulnerable to altered climates, along with how specific invasive species’ are responding to an altered climate regime.

These same authors provide specific recommendations to the global conservation community to put in place a more holistic perspective. Some recommendations deal with data integration. Others call for major undertakings: i.e., developing a protected area management toolkit at a global scale. This action will require significant investment in capacity-building of protected area managers plus international cooperation and technology transfer (Target 20). Hulme et al. suggest funding this effort should be a priority for any resources leveraged from international finance (Target 19).

Hulme et al. also propose changes in the conservation approaches advocated by the CBD and IUCN. Specifically, they call for more explicit consideration of current and future impacts of bioinvasions and their management — on protected areas. The needed activities fall into six areas:

(1) reduce risks associated with various pathways;                                 

(2) plan for range-shifting invasive species;

(3) mitigate invasive species’ impacts on biodiversity and (4) on ecosystem services;

(5) ensure new protected areas (including urban green spaces and infrastructure corridors) are largely free of established (“legacy”) invasive species; and

(6) provide managers sufficient resources to take effective action.

SOURCES

Fenn-Moltu, G., S. Ollier, O.K. Bates, A.M. Liebhold, H.F. Nahrung, D.S. Pureswaran, T. Yamanaka, C. Bertelsmeier. 2023. Global flows of insect transport & establishment: The role of biogeography, trade & regulations. Diversity & Distributions DOI: 10.1111/ddi.13772

Hulme, P.E., Lieurance, D., Richardson, D.M., Robinson, T.B. 2025 Multiple targets of Global Biodiversity Framework must be addressed to manage invasive species in protected areas. NeoBiota 99: 149–170. https://doi.org/10.3897/neobiota.99.152680

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at http://treeimprovement.utk.edu/FadingForests.htm

Or
https://fadingforests.org

New way to learn what others are doing … & tell them about your work!

field surveys; photo by F.T. Campbell

Several bioinvasion scientists have announced launch of a bi-annual Invasions Newsletter.  It will be an open-access digital magazine intended to meet the growing need for effective communication across the diverse community of researchers, practitioners, & policymakers. It will offer accessible insights into current research; communication & management strategies; novel technologies; research centers, groups, journals, networks, projects & resources; emerging policy trends; & past & upcoming meetings & events.

The initial issue is available here Among the topics addressed:  

  • invasive plant biocontrol efforts in Zimbabwe,
  • setting national-level invasive species priorities in Chile,
  • conservation actions to recover invaded endemic forests in Galápagos Islands,
  • protecting ground-nesting birds from introduced predators,
  • IUCN ISSG’s assistance in tackling invasive species in Europe.

The organizers — Ana Novoa, Susan Canavan, Katelyn T. Faulkner, Piero Genovesi,  Deah Lieurance, Dan Simberloff, Hsiao-Hsuan Wang, Tsungai Zengeya, & Laura A. Meyerson – invite us to contribute to future editions. Inform your global colleagues about your efforts and findings: fieldwork, model development, designing or implementing management interventions at a local, national or continental scale, or crafting policy frameworks.

outreach

To submit a contribution, contact any of the organizers.

Let’s ensure that tree-killing critters (with or without legs) get the attention they deserve!

Faith Campbell

Remote sensing – a promising ED method?

ash killed by EAB; photo by Nate Siegert, USFS

Scientists at the University of Minnesota have begun a project to assess the usefulness of remote sensing to detect the presence of emerald ash borer (EAB) earlier in the invasion. Previous studies had suggested that EAB infestation reduces leaf photosynthesis and transpiration before the yellowing of leaves. Scientists can monitor these changes from space. The project is now testing whether such monitoring can reliably detect EAB infestations at an early stage … The project began in April 2025 and is scheduled to end in December 2028.

Specific research questions to be addressed are:

  • How effective is remote sensing in detecting EAB years ahead of crown dieback?
  • Do changes in photosynthesis and transpiration caused by climate stresses (e.g. droughts and floods) differ from those caused by EAB infestation?
  • How quickly does an EAB infestation progress and spread spatially?

If remote sensing proves to be useful, land managers will have a new tool allowing them to intervene early enough to treat ash trees, before it is too late. The project team will build on existing detection protocols in collaboration with the USDA Forest Service, Minnesota Department of Agriculture (MDA), and Minnesota Department of Natural Resources (DNR).

I note that the Pacific coast states would benefit greatly from being able to identify satellite EAB outbreaks.

ash-dominated swamp in the Ankeny National Wildlife Refuge along the Willamette River in Oregon; photo by Wyatt Williams, Oregon Department of Forestry

I hope that this tool might also be tested for efficacy re: the non-native wood-borers attacking oaks and other trees in the Pacific coast states, e.g. goldspotted oak borer, Mediterranean oak borer, and three species of invasive shot hole borers.

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at  https://treeimprovement.tennessee.edu/

or

www.fadingforests.org

Help Detect Tree-killing insect in Southern California

Coast live oak killed by GSOB at William Heise State Park, San Diego County; photo by F.T. Campbell

Forest entomologists in southern California have organized the first of what they intend to be annual an annual “GSOB blitz”. The goldspotted oak borer has established widely in the region and has killed tens of thousands of California black and coast live oaks. 

The goal of the “blitz” is to train community members & organizations in detecting and reporting presence of this beetle. Survey events are scheduled in six Southern California Counties between June 1-June 15, 2025. Participants are welcome from the general public, private business, public or community organizations, etc.

Please join! & inform your friends!

To register for these training sessions, go to GSOB Blitz | UC Agriculture and Natural Resources

Shothole borer & associated fungus – demonstrating threat in South Africa & possibly beyond

Erythrina caffra one of the native tree species in South Africa killed by PSHB. photo by Coana/Riti via Flickr

Introductions of bark and ambrosia beetles (Coleoptera: Curculionidae, Scolytinae) have significantly increased over the past century. Surveys conducted at borders and ports of entry around the world have shown the majority of beetles intercepted were scolytines. These insects are highly destructive on their own. Also, they can carry pathogenic fungal symbionts that can have devastating effects on the trees they attack.

One or more species in a complex in the Euwallacea genus have become established in countries around the world.  One of these, the polyphagous shot hole borer (Euwallacea fornicatus; PSHB) and its associated fungus (renamed from Fusarium euwallaceae to Neocosmospora euwallaceae) is threatening havoc in South Africa about a decade after its establishment (Townsend, Hill, Hurley, and Roets. 2025).

Over this brief period PSHB/Fusarium disease has spread from two introduction sites – Pietermaritzburg, in KwaZulu-Natal Province, and Cape Town, in Western Cape Province – to all but one of the country’s nine provinces. It has become established in four of five forest types studied – Afrotemperate, coastal, sand, and swamp forests. It has not established in mangrove forests. (The Western Cape Province is home to its own “floral kingdom”. The kingdom’s charactersitic fynbos flora is a heathland habitat, not a forest one.)

Townsend and colleagues established a network of 78 monitoring plots in the Western Cape and KwaZulu-Natal provinces. The sites reflected a variety of natural and human impacts.

tree infested by PSHB/Fusarium disease in KwaZulu-Natal Botanical Garden, Pietermaritzburg. Photo from website of Greenpop.org

By monitoring these plots over five years (2019 – 2024), Townsend and colleagues have demonstrated that the beetle/fungus complex and resulting “Fusarium disease” is spreading and intensifying. The number of infected trees rose from 100 to 176 over the five years – a mean increase of 0.6% per year. The number of PSHB entry holes increased by over 10% annually. The number of plots containing infected trees roughly doubled from 23 in 2019 (29% of the 78 plots) to 48 (60%) in 2023.

By the end of the study, 29% of the 148 species sampled had been infected. This represented 43 species and 7 unidentified trees infected. Trees of eight native species died, , although one — Diospyros glabra (Ebenaceae) – resprouted after the main bole died.

In addition to the eight species known to suffer mortality, another 18 species were found to be able to support PSHB reproduction. Townsend and colleagues worry that, as the infestation spreads and intensifies, some of these species might also succumb. They mention specifically Erythrina caffra (coral tree), which is prevalent in coastal forest ecosystems across South Africa.

Most of the hosts are in the same families as those identified earlier by Lynch et al. (2021), e.g., Ebenaceae, Fagaceae, Fabaceae, Malvaceae, Podocarpaceae, Rutaceae, Sapindaceae and Stilbaceae.

Disease progress, speed of death, and visibility of symptoms varied not only between species, but sometimes among individuals of the same species. Some trees died rapidly. Townsend and colleagues say it is impossible to predict which individuals will succumb to infection.

There is, though, a clear frequency-dependent relationship between trees and beetles. Sites with higher relative abundance of host trees also had a higher proportion of infected trees, on average. The number of PSHB holes per species and per plot both increased to a larger extent at these same sites.

Individual trees’ traits influenced the severity of infestations (measured by the number of PSHB entry holes). Larger trees, those with a less healthy canopy, and those farther from a water source suffered more attacks. (This last finding differs from others’; Townsend et al. speculate that in the absence of flood-stressed trees, drought-stressed trees might be more attractive to ambrosia beetles.)

native tree in Tsitsikama National Park; photo by F.T. Campbell

Characteristics of the monitoring plots also affected disease progression. Higher proportions of trees became infected when they grew in plots that were closer to source populations, or that contained a higher proportion of host species as distinct from non-host species. The proportion of trees infected decreased in plots with higher tree densities or tree species richness.

As of 2023, “Fusarium disease” is more widespread and intense in KwaZulu-Natal than in the Western Cape. In KwaZulu-Natal 0.11% of monitored trees are infected compared to 0.06% in the Western Cape. The number of infected trees rose twice as fast over the five years in KwaZulu-Natal – ~6%, than in Western Cape – 3%. While all KwaZulu-Natal plots contained infected trees, three of 11 monitoring sites in the Western Cape did not. Townsend and colleagues believe that the most likely explanation is that PSHB arrived in KwaZulu-Natal earlier (as far back as 2012 as opposed to 2017 in Western Cape). Another possible factor is that source populations of infected trees are indigenous trees within the forest in KwaZulu-Natal whereas, in the Western Cape, they are often non-native trees planted in urban areas far from the study plots. Also, forests in KwaZulu-Natal are fragmented while, in Western Cape, the study forests are nearly contiguous. Townsend et al. conclude that the disease will spread and intensify in Western Cape as additional source populations become established in the forest.

locations of PHSB/Fusarium disease in Cape Town, South Africa – West of the study sites; map from City of Cape Town

As of 2023, the proportion of trees infected appears to be small — 7.6% of the 2,313 trees monitored. Only 11 trees in the monitored plots have died. However, the longer PSHB is active in the environment the more trees it will infest, the higher its impact will be on hosts, and the higher the number of dispersing individuals produced. This will substantially increase the chances and rates of additional areas becoming infected, especially in areas close to infestations – e.g., cities. They fear that in the future impacts will increase as progressively more competent host individuals are infected. Therefore, they emphasize the importance of mitigating PSHB increase in natural ecosystems, even in already infected areas.

Townsend and colleagues urge phytosanitary officials and resource managers to prioritize surveillance and management on the families containing several host species (above) and within plant communities in which they predominate. Managers must also be alert to new reproductive hosts for the beetle that appear as the infestation spreads and intensifies.

The situation could be worse than described; the Townsend et al. study did not examine how the invasion might affect eco-regions outside these two provinces. Because the PSHB has such a broad host range, hosts can die quickly, and South Africa provides ideal climatic conditions, this bioinvader could cause severe ecological effects on most indigenous forest types as well as agriculture and urban trees throughout Africa.

SOURCES

Lynch, S.C., A. Escalen, and G.S. Gilbert. 2021. Host evolutionary relationships explain tree mortality caused by a generalist pest-pathogen complex. Evol Appl 14:1083 – 1094. https://doi.org/10.1111/eva.13182

Townsend, G., M. Hill, B.P. Hurley, and F. Roets 2025. Escalating threat: increasing impact of the polyphagous shot hole borer beetle, Euwallacea fornicatus, in nearly all major South African forest types. Biol Invasions (2025) 27:88 https://doi.org/10.1007/s10530-025-03551-2  

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at  https://treeimprovement.tennessee.edu/

or

www.fadingforests.org

“Ecological memory” determines a forest’s resilience — implications of bioinvasion to New Zealand’s unique flora

kauri dieback

Scientists in New Zealand are saying explicitly that a forest’s unique mixture of species matters when considering the future. This mixture is the result of the forest’s evolutionary history. Losing members of the biological community reduces the forest’s ability to respond to current and future stresses – its resilience.

New Zealand’s forests are part of the broader legacy of the ancient supercontinent of Gondwanaland – the island nation’s plants have close relatives in South America, the Pacific Ocean islands, and Australia. Still, these forests are unique: 80% of New Zealand’s plant species are endemic. The forests are also species-rich. The warm temperate evergreen rain forests of the North Island are home to at least 66 woody plant species that can reach that reach heights above six meters (Simpkins et al. 2024).

These forests have been severely changed by human activity. In just ~ 750 years people have cut down approximately 80% of the original forest cover! (Simpkins et al. 2024) Of the eight million hectares of surviving native forest, a little over five million hectares is managed for the conservation of biodiversity, heritage, and recreation.  Another 2 million hectares are plantations of non-native species.

sites in New Zealand where pine plantations are “wilding”

All these forests are challenged by introduced mammals – from European deer to Australian possums. Climate change is expected to cause further disturbance, both directly (through e.g., drought, extreme weather) and indirectly (e.g., by facilitating weed invasion and shifting fire regimes) (Simpkins et al. 2024).

Pathogen threats are also common threats to the native trees of the Pacific’s biologically unique island systems. For example, Ceratocystis lukuohia and C. huliohia (rapid ‘ōhi‘a death, or ROD). The latter is killing ‘ōhi‘a (Metrosideros polymorpha) on the Hawaiian Islands. More than 40% of native plant species in Western Australia are susceptible to Phytophthora cinnamomi. Here I focus on two pathogens, kauri dieback and myrtle rust, now ravaging New Zealand’s native flora. No landscape-level treatment is available for either pathogen.

When considering this suite of challenges, Simpkins et al. focus on these two pathogens’ probable impact on forest carbon sequestration. They worry in particular about erosion of the forests’ resilience due to loss of “ecological memory” – the life-history traits of the species (e.g., soil seed banks) and the structures left behind after individual disturbances.

one of the largest remaining kauri trees, “Tane Mahuta”, in Waipoua Kauri Forest; photo by F.T. Campbell

Kauri Dieback

The causal agent of Kauri dieback, Phytophthora agathidicida, is a soil-borne pathogen that spreads slowly in the absence of animal or human vectors. The disease affects a single species, Agathis australis (kauri, Araucariaceae). However, kauri is a long-lived, large tree that is a significant carbon sink. It probably modifies local soil conditions, nutrient and water cycles, and associated vegetation. Also, kauri has immense cultural significance.

Simpkins et al. note that kauri dieback threatens stand-level loss of A. australis – that is, local extinctions. In the absence of disturbance Kauri trees can grow to awe-inspiring size. In the 19th Century, before widespread logging, some were measured at 20 meters or more in circumference. Consequently, kauri dieback might cause a decline in aboveground live carbon storage of up to 55%. This loss would occur over a period of hundreds of years, not immediately.

Huge kauri are not likely to be replaced by other long-lived emergent conifers (based on an analysis of one species, Dacrydium cupressinum). Instead, kauri are probably going to be replaced by late-successional angiosperms. The authors discuss the ecological implications for levels of carbon storage and proportions of trees composed of Myrtaceae – exacerbating damage caused by myrtle rust (see below).

The expectation of Simpkins et al. that kauri will suffer at least local extinctions is based on an assumption that no kauri trees are resistant to the pathogen. Fortunately, this might not be true: different Agathis populations show various levels of tolerance to Agathis dieback. Identification and promotion of some levels of resistance could enable A. australis to retain a diminished presence in the landscape.

However, Lantham, et al. make clear that containing kauri dieback remains “challenging,” despite its discovery nearly 20 years ago (in 2006). Scientists and land managers have little information on the distribution of symptomatic trees, much less of the pathogen itself. This means they don’t know where infection foci are or how fast the disease is spreading.

As is often true, the pathogen is probably present in a stand for years, possibly a decade or more, before symptoms are noticed. This means that the current reliance on public reports of diseased trees, or targetting surveillance on easy-to-access sites (e.g., park entrances and along existing track networks), or at highly impacted areas readily identified through aerial methods, fails to detect early stages of infection. Indeed, it seems probable that P. agathidicida had been present in New Zealand’s ecosystems for decades before its formal identification.

The Waipoua forest is one of the largest areas of forest with old kauri stands in the country. A new analysis of aerial surveys done between 1950 and 2019, shows how the forest is changing. The number of dead trees increased more than four-fold and the number of unhealthy-looking trees increased 16-fold over these 70 years. Kauri dieback is now widespread in this forest, especially in areas near human activities like clearing for pasture or planting commercial pine plantations).

Lantham et al. have developed a model which they believe will help identify areas of higher risk so as to prioritize surveillance and inform responses. These could delimit the disease front and help implement quarantines or other measures aimed at limiting the spread of P. agathidicida to uninfected neighboring sites.

I hope New Zealand devotes sufficient resources to expand surveillance and management to levels commensurate with the threat to this ecologically and culturally important tree species.

Leptospermum scoparia; photo by Brian Gatwicke via Flickr

Myrtle Rust

Myrtle rust is a wind-borne disease that affecting numerous species in the Myrtaceae, including some of the dominant early successional species (e.g., Leptospermum spp.). Simpkins et al. expect that myrtle rust might hasten the decline of two such tree species (L. scoparium and Kunzea ericoides). However, these trees’ small size and rapid replacement by other species during succession minimizes the effect of their demise on carbon storage.

Because I am concerned about the irreplaceable loss to biodiversity, I note that Simpkins et al. also feared immediate threats to some trees in the host Myrtaceae family, specifically highly susceptible species such as Leptospermum bullata.

As I reported in a recent blog, a second group of scientists (McCarthy et al.) explored the threat from myrtle rust more broadly. Austropuccinia psidii has spread through Myrtaceae-dominated forests of the Pacific islands for about 20 years.

Trees in the vulnerable plant family, Myrtaceae, are second in importance (based on density and cover) in New Zealand’s forests. Successional shrub communities dominated by the two species named above, Kunzea ericoides and Leptospermum scoparium, are widespread in the northern and central regions of the North Island and in northeastern and interior parts of the South Island. These regions’ vulnerability is exacerbated by the area’s climate, which is highly suitable for A. psidii infection (Simpkins et al. 2024).

McCarthy et al. concluded that if Leptospermum scoparium and Kunzea ericoides prove to be vulnerable to myrtle rust, their loss would cause considerable change in stand-level functional composition across these large areas. They probably would be replaced by non-native shrubs, which are already common on the islands. Any resulting forest will differ from that formed via Leptospermeae succession.

These authors also worry that the risk to native ecosystems would increase if more virulent strains of the myrtle rust pathogen were introduced or evolved. They note that A. psidii is known to have many strains and that these strains attack different host species.

SOURCES

Latham, M.C., A. Lustig, N.M. Williams, A. McDonald, T. Patuawa, J. Chetham, S. Johnson, A. Carrington, W. Wood, and D.P. Anderson. 2025.  Design of risk-based surveillance to demonstrate absence of Phytophthora agathidicida in New Zealand kauri forests. Biol. Invasions (2025) 27, no. 26

McCarthy, J.K., S.J. Richardson, I. Jo, S.K. Wiser, T.A. Easdale, J.D. Shepherd, P.J. Bellingham. 2024. A Functional Assessment of Community Vulnerability to the Loss of Myrtaceae from Myrtle Rust. Diversity and Distributions, https://doi.org/10.1111/ddi.13928

Simpkins, C.E., P.J. Bellingham, K. Reihana, J.M.R. Brock, G.L.W. Perry. 2024. Evaluating the effects of two newly emerging plant pathogens on North Aotearoa-New Zealand forests using an individual-based model.  Ecological Modelling, www.elsevier.com/locate/ecolmodel

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at  https://treeimprovement.tennessee.edu/

or

www.fadingforests.org

More pests in Europe & Mideast – hazard to North American trees

giant sequoia; photo by Matthew Dillon via Flickr

The pest alert system “PestLens” has again alerted us to plant pests in Europe or Asia that feed on species closely related to tree species native to North American forests.  Two of the insects named in the alert apparently pose a hazard to icons of the forests of America’s Pacific coast forests, giant sequoia and redwood.

I hope APHIS is using this information to alert port and on-the-ground staff and perhaps initiating more in-depth risk assessments.

The posting on February 27, 2025 reported that cotton jassid, Jacobiasca lybica (Hemiptera: Cicadellidae), affects not just cotton and citrus but also Cupressus sempervirens (Mediterranean cypress) [Cupressaceae]. More than a dozen North American trees species are in this family, including

  • Sequoiadendron giganteum or giant sequoia. Giant sequoia is listed as an endangered species by the IUCN with fewer than 80,000 remaining in its native California.
  • Chamaecyparis thyoides and C. lawsoniana (Port-Orford cedar). Port-Orford cedar has been decimated in its native range by an introduced pathogen, Phytopthora lateralis. A major breeding effort has developed trees that are resistant to the pathogen; they are now available for people to plant.
  • Thuja occidentalis, also known as northern white-cedar, eastern white-cedar, or arborvitae,
  • Taxodium ascendens, also known as pond cypress
  • several Juniperus
  • Hesperocyparis macrocarpa also known as Cupressus macrocarpa, or the Monterey cypress. NatureServe ranks the cypress as GI – critically imperiled.

Cotton jassid been reported from several countries in Europe, Africa, and the Middle East.

China has reported the existence of a previously unknown bark beetle species, Phloeosinus metasequoiae (Coleoptera: Curculionidae). It was found infesting Metasequoia glyptostroboides (dawn redwood) trees in China. Affected trees exhibited reddened leaves and holes and tunnels in branches.

China has also discovered a several new hosts utilized by the fungus Pestalotiopsis lushanensis (Sordariomycetes: Amphisphaeriales). Formerly known to infect tea (Camellia sinensis) and several other plant species, P. lushanensis has now been found shoot causing blight and leaf drop on a conifer, deodar cedar (Cedrus deodara) and leaf spots on an angiosperm with congeners in North America — the rare Chinese species, Magnolia decidua. There are eight species of Magnolia native to North America.

Magnolia grandiflora; photo by DavetheMage via Wikimedia

APHIS’ ability to respond to alerts remains uncertain.

The agency’s probationary employees have been fired – just as at other agencies. APHIS staff were prohibited from participating in last week’s annual USDA Invasive Species Research Forum – the 33rd such meeting. The bird flu emergency is demanding all the attention and funds.

So – how can the rest of us fill in?

At the USDA Research Forum I again presented a poster urging greater attention to tree-killing pathogens. Scientists have made considerable progress in identifying factors that indicate whether a non-native insect might pose a significant threat (see blogs on conifer and deciduous species; more to come!). However, USDA had not funded a similar effort to improve understanding of pathogens. The most promising strategy so far are sentinel plantings. However, these systems have weaknesses; I will blog in the near future about another analysis.

I propose that APHIS start by working with independent scientists to determine the actual, current level of pathogens associated with various types of incoming goods. Contact me directly if you wish to read the text of my poster.

Posted by Faith Campbell

We welcome comments that supplement or correct factual information, suggest new approaches, or promote thoughtful consideration. We post comments that disagree with us — but not those we judge to be not civil or inflammatory.

For a detailed discussion of the policies and practices that have allowed these pests to enter and spread – and that do not promote effective restoration strategies – review the Fading Forests report at  https://treeimprovement.tennessee.edu/

or

www.fadingforests.org